

Introduction
Despite the significant potential of NPs in agriculture, few products are currently available. Here are a few examples of available or promising nanoproducts in agriculture, e.g., nano-insecticides, nano-pesticides, nano-fertilizers, Nano-encapsulation of bioactive compounds, Nano-sensors and precision agriculture, and Nano-delivery systems. This is partially due to concerns about their potentially harmful effects on living organisms and the potential for contamination of agricultural lands, water resources, and air pollution. Therefore, before NPs use, lab-scale studies should be conducted on plants to investigate their impacts, including uptake, translocation, and cellular import, as well as interactions between cells and NPs. Additionally, examining plant responses to NP applications at the physiological, biochemical, and molecular levels may provide insights into the plants’ health status [1-4]. Studies have shown that nanoparticles (NPs) can impact the morphological features of plants and the intensity of photosynthesis [5-10]. The effect on plants can be positive or negative, and it depends on the size, concentration, and type of NPs [11-14]. Pariona et al. showed that application of Fe3O4 NPs decreased plant growth in Quercus macdougallii [1]. Fe3O4 NPs prevented leaf expansion and germination of wheat (Triticum vulgare Vill) [9,]. Fe-NPs positively influenced seed germination and seedling growth of wheat under dehydration and salinity in Triticum Vulgare [14], and Triticum Aestivum [15]. Fe3O4 Nanoparticles protected seeds during the germination of Cucumis Sativus [16]. Iron Oxide Nanoparticles influenced wheat (Triticum Aestivum L.) development [17]. The impact of nanoparticles on plant growth was documented for many plant species, especially fenugreek (Trigonella foenum-graecum L.) [18], rice (Oryza sativa L.) [19], sunflower (Helianthus annuus L.) [20], and barley (Hordeum vulgare L.) [21].
The purpose of the study was to determine how Fe3O4 NPs affected the seed germination of beans and seedling growth. GPOX and ADH activities were determined. We hypothesize that improvements in plant production after treatment with Fe3O4 NPs are related to the stimulation of antioxidant systems and metabolism processes during the early stages of seedling establishment.
Material and Methods
Particle size quantification: Particle size quantification of Fe3O4 NPs stock suspension was determined by dynamic light scattering (DLS) using a Malvern (zetasizer nano-ZS) particle analyzer, and this analysis demonstrated an average particle size of Fe3O4 NPs1 about 43 nm and Fe3O4 NPs2 about 6 nm in the 50 µg L−1 stock, respectively, for Fe3O4 NPs synthesized by co-precipitation and green synthesis processes.
Plant material and growth conditions: Genotype tested comprised white beans (Phaseolus vulgaris L. Snowdon) from Saudi Arabia, disinfected with 2% sodium hypochlorite for 10 min, rinsed thoroughly, and soaked in distilled water at 4 °C for 24 h. Five seeds were germinated on 9-cm diameter Petri dishes containing two sheets of filter paper moistened with 10 mL distilled water (for control) or two concentrations of Fe3O4 NPs (0.05 or 0.1 mg mL-1) at 25 °C in the dark for 6 days. Fe3O4 NP preparations were dispersed by ultrasonic treatment for 60 min and maintained in the dark. At harvest, the embryonic axes and cotyledon were weighed and stored in liquid nitrogen until analysis or dried for 8 days at 70 °C for dry weight determination. In the laboratory stage, an experiment was conducted with six replicas, and each Petri dish contained ten seeds.
Non-enzymatic antioxidant extraction: Cotyledons and embryonic axes of bean (0.5 g) were powdered and homogenized with 5 mL of 80% ethanol, boiled for 30 min at 60 °C, and then centrifuged at 8000×g for 10 min at 4 °C. The supernatants were used as samples to determine total soluble sugars and amino acids.
Determination of soluble sugars content: In an acidic medium, soluble sugars are dehydrated to furfural compounds, which are condensed in the presence of anthrone in colored products. 30 μL of supernatants are added to 0.5 mL of distilled water and 2 mL of 0.2% anthrone solution (prepared in concentrated sulfuric acid). The mixture is stirred in a boiling water bath for 15 min and then cooled on ice for 5 min. The intensity of the coloring solution was measured using a spectrophotometer at 625 nm. A standard sucrose was used for calibration [22].
Determination of amino acids content: The free amino acids are deaminated by ninhydrin, releasing ammonia, which reacts with ninhydrin to form a colored compound. To 30 µL of ethanoic extracts are added 300 µL of 0.9 M citric acid, pH 5.2, and 600 µL of a solution of ninhydrin 1.5% (prepared hot in a 60% ethanol/H2O mixture, V/V, in the presence of 40 mg of ascorbic acid). After stirring, incubation in a boiling water bath for 15 min, and rapid cooling on ice, 2 ml of 60% ethanol are added. The optical density is then measured at 570 nm [22].
Fig. 1.
Germination rate of bean (Phaseolus vulgaris) seed after imbibition with H2O, Fe3O4 NPs1 or Fe3O4 NPs2 after six days. Data are means (±SE) of four replicates with one seedling each. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
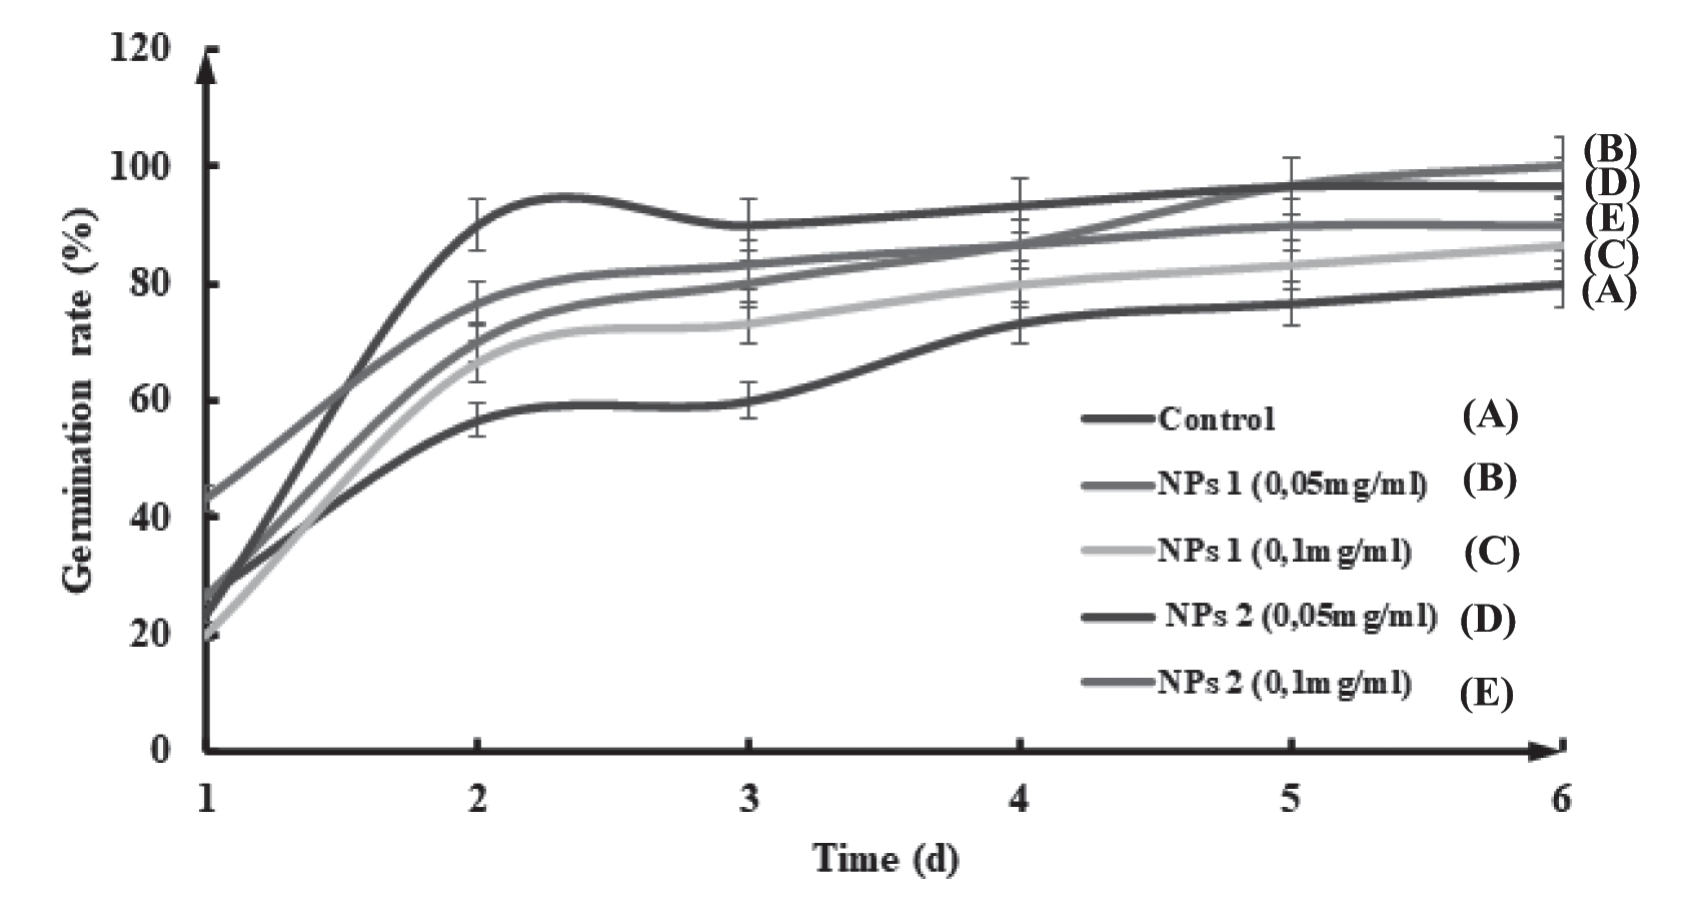
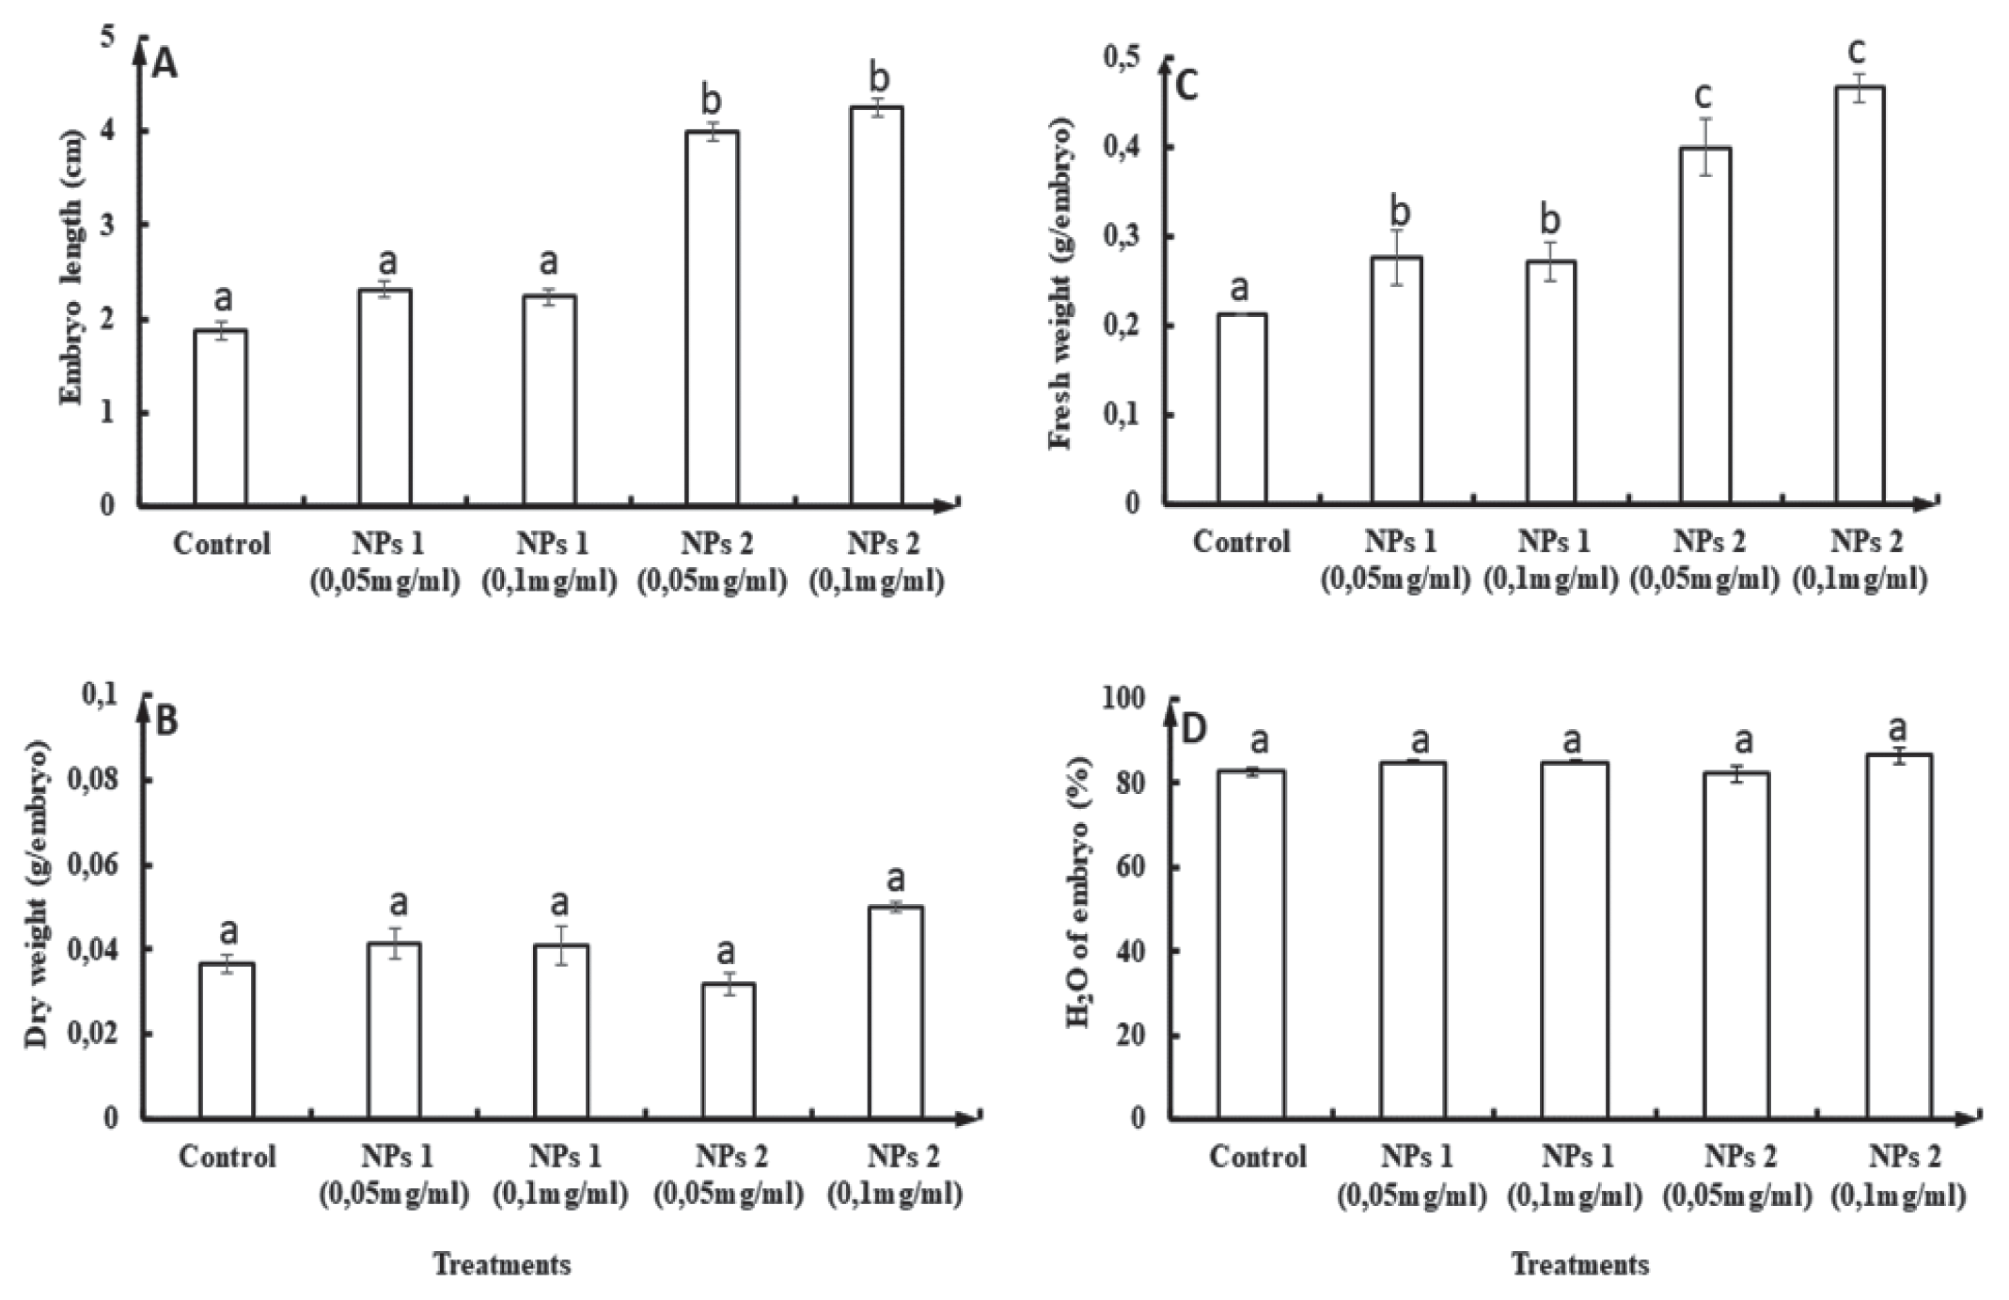
Fig. 2.
Embryo length (A), dry weight (B), fresh weight (C), and water content (D) of embryonic axis of bean (Phaseolus vulgaris) seed after imbibition with H2O, Fe3O4 NPs1 or Fe3O4 NPs2 after six days. Data are means (±SE) of four replicates with one seedling each. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
Electrolyte leakage: The germination medium was analyzed for electrolyte leakage. The filter paper was carefully folded and compressed to remove the majority of the medium solution. In order to measure electrolyte leakage, a conductivity meter (Model 250, Denver Instrument) was used. Based on the seed number, the electrical conductivity was expressed. Blanks containing water or solutions of nanoparticles were included. Each treatment consisted of five replicates, and each experiment was carried out at least twice [22].
Determination of guaiacol peroxidase (EC 1.11.1.7) activities: Fresh tissues were ground with a mortar in a homogenization medium (w/v =1/3) (pH 7.5) consisting of Tris-HCl (50 mmol L-1), saccharose (0.4 mol L-1), and EDTA-Na2 (5 mmol L-1). The homogenate was centrifuged at 800×g for 5 min. The resulting supernatant was centrifuged again at 20.000×g for 30 min. The chloroplast pellet was suspended in the homogenization medium and kept at 4°C [23]. Guaiacol peroxydase activity was measured following the H2O2-dependent oxidation of guaiacol according to the protocol described by Missaoui et al. [8]. The enzyme extract was added to the reaction mixture, which contained 50 mM of potassium phosphate (pH 7.0), 10 mM of H2O2, and 9 mM of guaiacol. The enzyme activity was estimated by the increase in absorbance at 470 nm using a UV-visible spectrophotometer (Lamba 2, PerkinElmer). The GPOX activity was determined using the extinction coefficient of 26.6 mM-1 cm-1.
Determination of alcohol dehydrogenase (EC 1.1.1.1) activities: Fresh tissue was ground in a mortar and pestle in 50 mM KH2PO4 (pH 7.5) containing 0.4 M sucrose, 1 mM EDTA, 5 mM DTT, and 2% BSA (1 :2. W : V). The homogenate was squeezed through double cheesecloth and centrifuged at 20.000 × g for 20 min. The supernatant obtained was carefully decanted and used for alcohol dehydrogenase (ADH) assays. All procedures were carried out at 4°C [24].
Statistical analysis: All data were statistically analyzed using two-way ANOVA, and the means were separated using the Newman–Keuls multiple-range test (Statistica 8, StatSoft Co., USA). Differences were considered significant at p<0.05.
Results and Discussion
Germination is essential for effective plant establishment. As a critical stage in a plant’s life cycle, germination is influenced by environmental conditions, including temperature, salinity, light, soil moisture, and nanoparticle exposures [25-29]. 50 mg/L of Fe3O4 NPs1 did not affect the seed germination of the bean. However, 100 mg/L Fe3O4 NPs1 and Fe3O4 NPs2 stimulated germination rates (Fig. 1).
The dose of nanoparticle, duration of treatment, method of application, type of nanoparticle, and plant species always have an impact on crop yield. In the case of Fe nanoparticles, they showed better results in improving nutrient uptake and germination [25,30,31]. The effects of Fe3O4 NPs1 and Fe3O4 NPs2 on the seed germination of the bean varied depending on several factors, such as the concentration of Fe3O4 NPs and the method of synthesis of Fe3O4 NPs. The results agreed with those from Tombuloglu et al. [32]. A study by Sathishkumar et al. [33] compared the effects of Fe3O4 NPs1 and Fe3O4 NPs2 methods on the germination of soybean seeds. The results showed that Fe3O4 NPs2 had a higher positive impact on seed germination and growth compared to the Fe3O4 NPs1.
Fe3O4 NPs2 increased embryo length by about 2-fold over six days (Fig. 2A). There were no differences between dry weight and water content for Fe3O4 NPs2- treated embryonic axis (Fig. 2B,D). Embryo fresh weights decreased by about 130% and 200% after six days of treatment with Fe3O4 NPs1 and Fe3O4 NPs2, respectively (Fig. 2C).
The reduction of plant biomass can be attributed to high concentrations of Fe3O4 NPs in apoplast, which can lead to clogging and limited water and nutrient absorption. Another possibility for the growth reduction is deformation or damage to vascular bundles due to the high dose effect of Fe3O4 NPs. In addition, the increase in plant biomass can be attributed to the formation and accumulation of OH radicals that cause cell wall loosening and cell elongation [1]. Fresh weights from Fe3O4 NPs2-treated cotyledon increased by about 150% over six days. Fresh and dry weights from cotyledons were slightly reduced after treatment with Fe3O4 NPs1 compared to control after 6 days (Fig. 3A,B). In addition, there were no differences in water content in cotyledon (Fig. 3C).
Fig. 4.
Electrical conductivity of germination medium of bean (Phaseolus vulgaris) after imbibition with H2O, Fe3O4 NPs1 or Fe3O4 NPs2. Values represent means (±SE) of cinq replicates. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
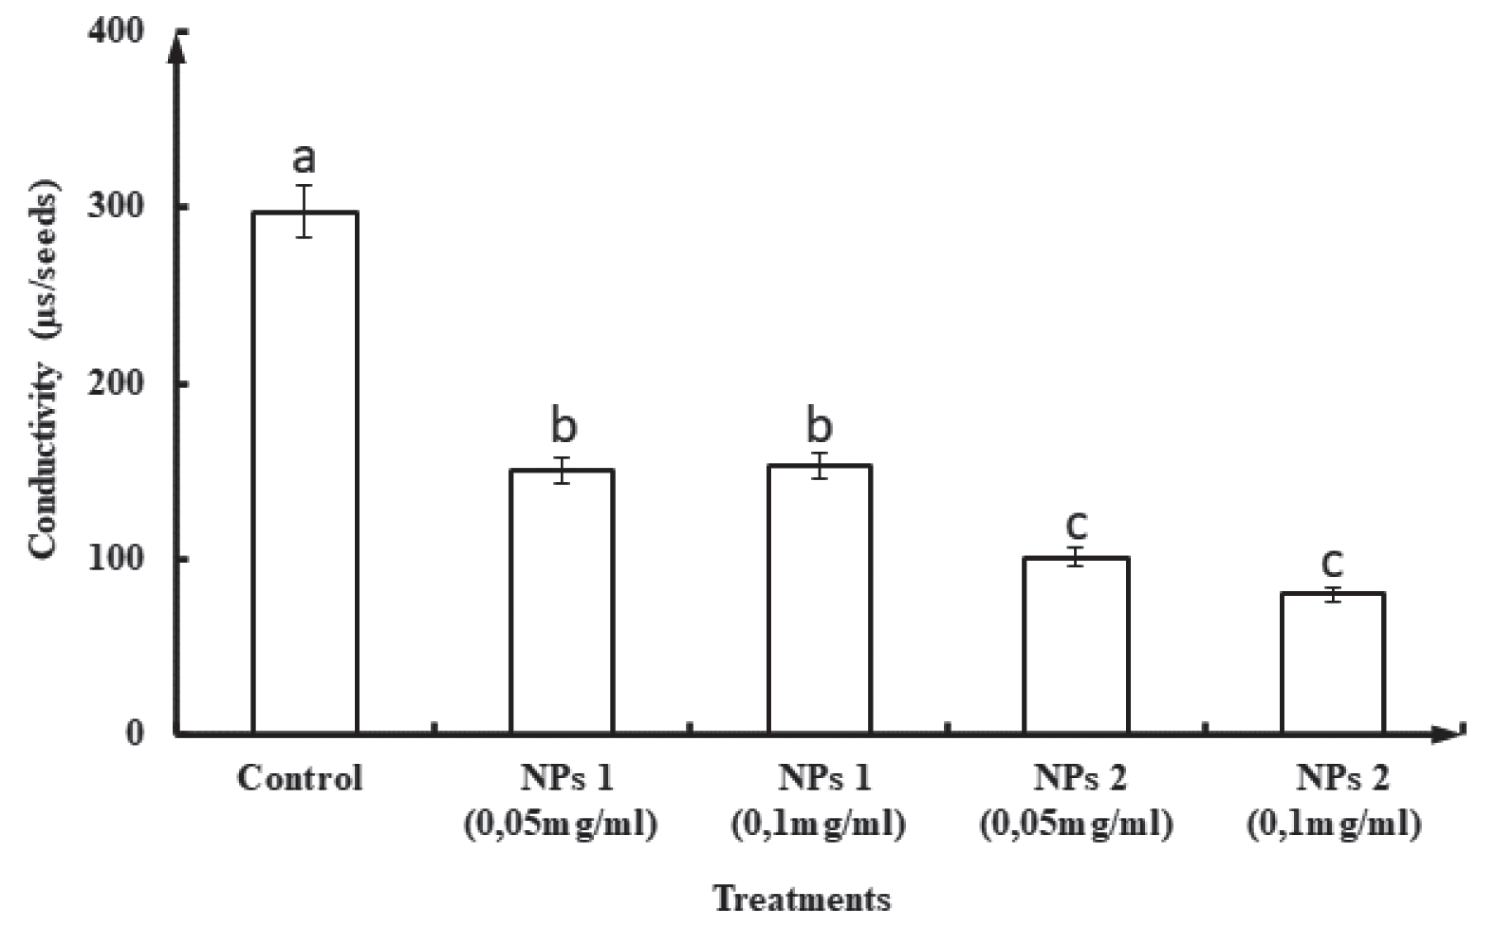
Fig. 3.
Fresh weight (A), dry weight (B), and water content (c) cotyledon of bean (Phaseolus vulgaris) seed after imbibition with H2O, Fe3O4 NPs1 or Fe3O4 NPs2 after six days. Data are means (±SE) of four replicates with one seedling each. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
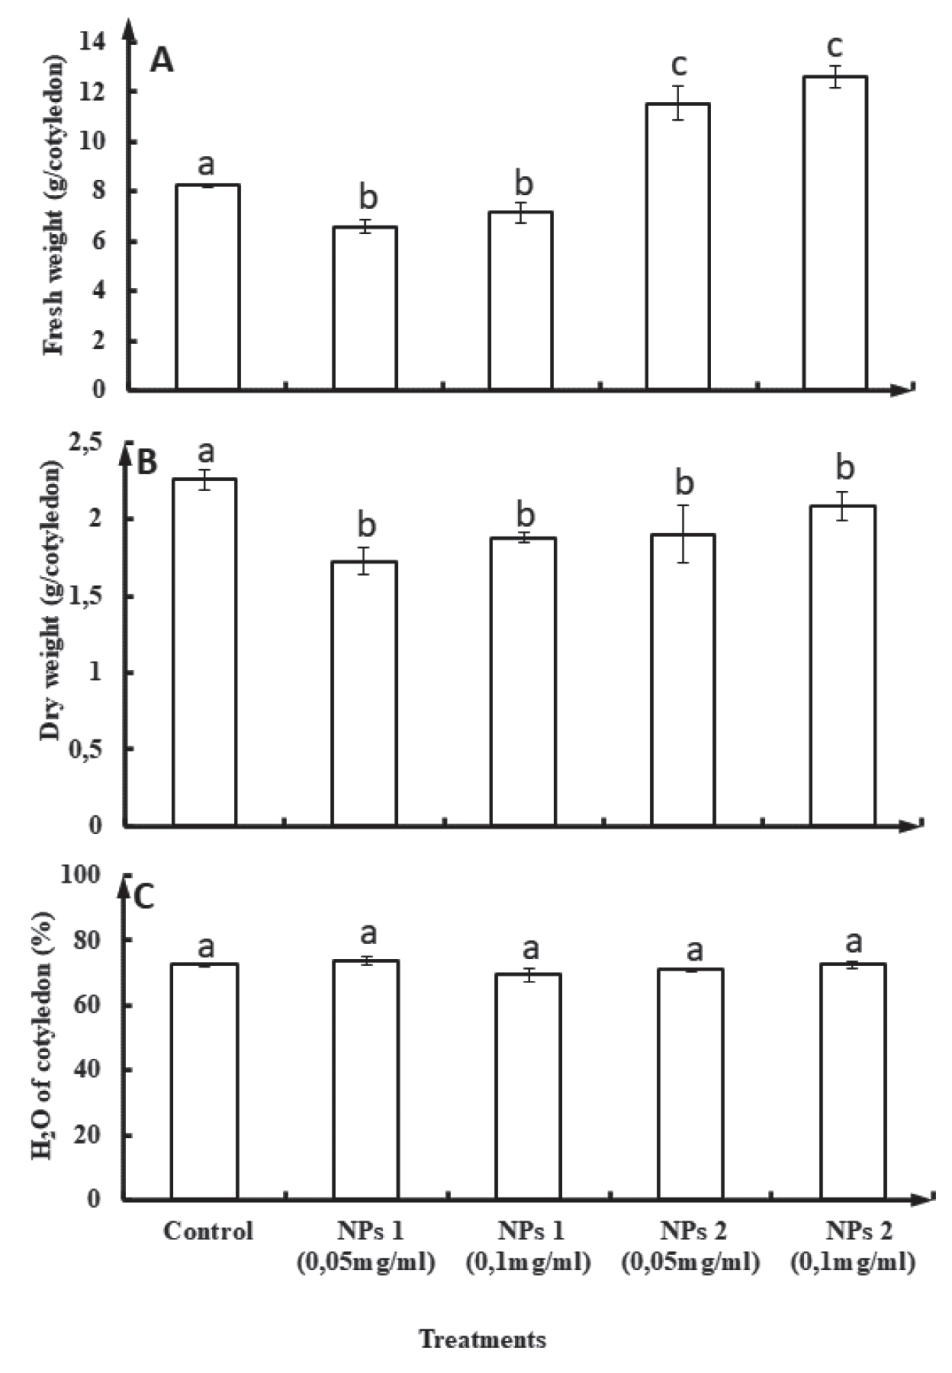
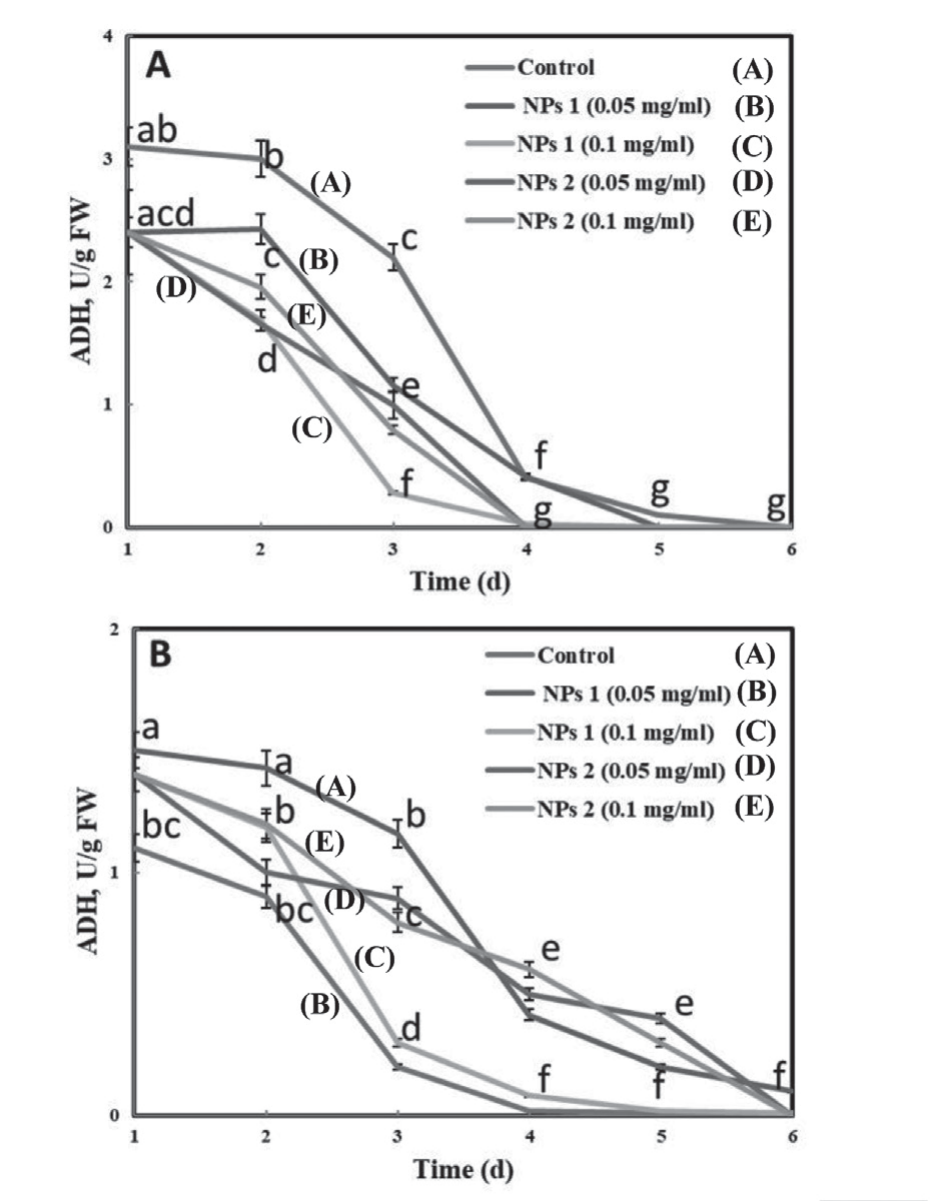
Fig. 5.
Effects of Fe3O4 NPs1 and Fe3O4 NPs2 on ADH in embryonic axis (A) and cotyledon (B) of bean (Phaseolus vulgaris) seedlings. Data are means (±SE) of four replicates. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
There was a reduction of about 75% and 77% in free amino acids and soluble sugar levels in embryonic axes treated with Fe3O4 NPs1. 50-100 mg/L Fe3O4 NPs2 reduced metabolite levels by about 20-55%, compared to control after 6 days (Table 1). In cotyledon, at 100 mg/L Fe3O4, Fe3O4 NPs1, and Fe3O4 NPs2 decreased soluble sugar and amino acids by about 50-66% and 20-55%, respectively. At 50 mg/L Fe3O4 NPs2 free amino acids and soluble sugars, levels were reduced by about 13-29%, respectively.
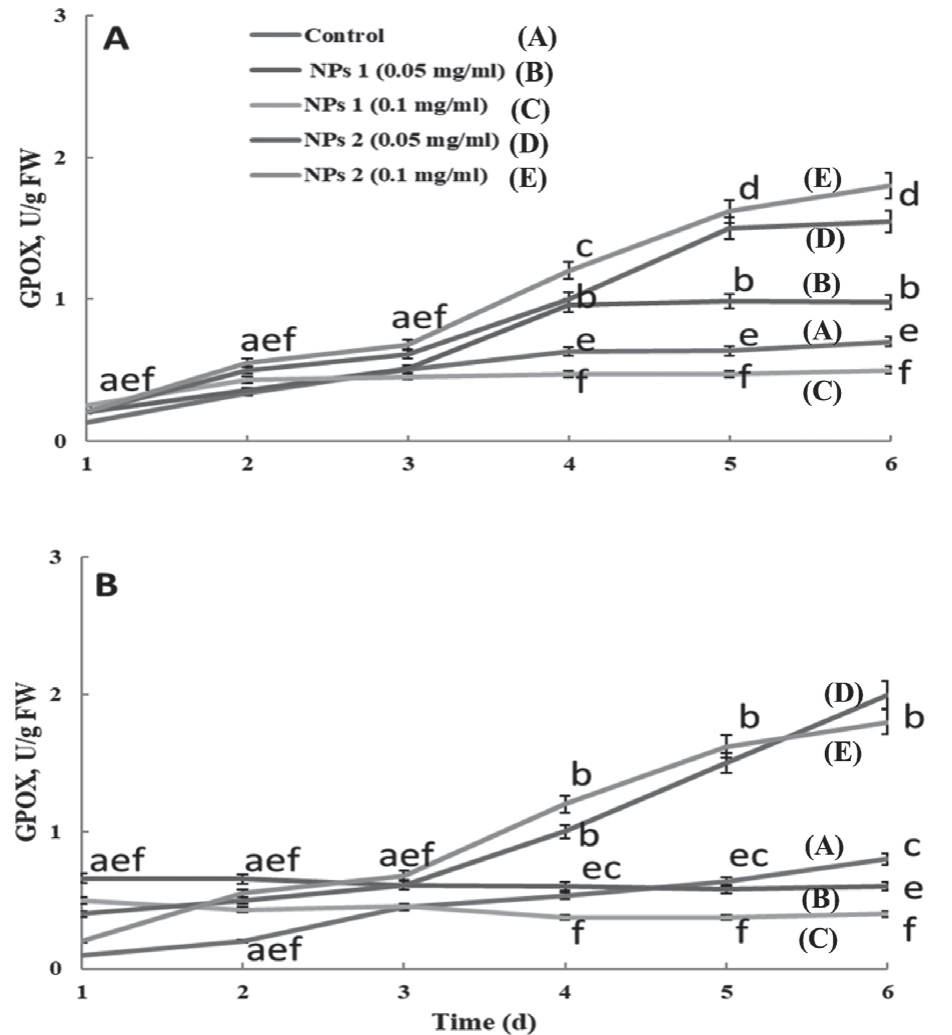
Fig. 6.
Effects of Fe3O4 NPs1 or Fe3O4 NPs2 on GPOX of embryonic axis (A) and cotyledon (B) of bean (Phaseolus vulgaris) seedlings. Data are means (±SE) of four replicates. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
Gupta et al. [30] suggested that the Fe3O4 NPs significantly increased starch, soluble proteins, soluble sugars, and oil content from seeds. The effects of Fe3O4 NPs on seed germination and growth depended on multiple factors related to nanoparticles, such as particle size, surface chemistry, and exposure time.
Table 1.
Soluble sugar and amino acids contents of bean (Phaseolus vulgaris) after imbibition with H2O, Fe3O4 NPs1 or Fe3O4 NPs2. Values represent means (±SE) of three replicates. Different letters represent significant differences between the treatment means. Differences were considered significant at P < 0.05 level.
Seeds imbibed with H2O have lower values of solute leakage. The values decreased by 50% and 34% for Fe3O4 NPs1 and Fe3O4 NPs2, respectively, compared to the control after 6 days of germination (Fig. 4).
The initial high activities of alcohol dehydrogenase (ADH) were declined in embryo axes and cotyledon and disappeared absolutely after four days of germination in seed imbibed with H2O. ADH activities in embryo axes Fe3O4 NP-treated seeds decreased significantly compared to control after 6 days of germination (Fig. 5A). However, Fe3O4 NP-treated cotyledons had significantly higher-level ADH activities compared to control (Fig. 5B). NP-treated seeds showed an increase in dehydrogenase activity and a decrease in solute leakage. Both measures are indicators for seed viability [34].
Antioxidant enzymes play a crucial role in protecting cells from oxidative stress, which can cause damage to cellular structures and biomolecules such as DNA, proteins, and lipids. There were several types of antioxidant enzymes, including catalase, superoxide dismutase (SOD), and peroxidase. These enzymes neutralized harmful reactive oxygen species (ROS) that were generated during germination or in response to environmental stressors [35, 36].
Application of 50 mg/L Fe3O4 NPs1 improved GPOX activities in embryo axis (40%) but inhibited them by about 28% with 100 mg/L compared to control after 6 days of germination. GPOX activities were highly stimulated by about 120-160% with Fe3O4 NPs2 (Fig. 6A). In cotyledon, Fe3O4 NPs1 decreased by about 25-50%, but Fe3O4 NPs2 induced activities by about 125-150% (Fig. 6B). In comparison with controls, plants treated with NPs showed greater antioxidant enzyme activities in both the root and aerial sections, indicating a change in defense mechanisms that reduced oxidative damage. These results show that Fe3O4 NPs are not phytotoxic, suggesting that they may be useful in the creation of innovative agricultural products [22, 37-39].
Conclusion
According to the research’s findings, Fe3O4 NPs induced the growth of bean seedlings (Phaseolus vulgaris). Dehydrogenase activities and solute leakage metabolisms-controlled seed viability during germination. Effects caused by the presence of Fe3O4 NPs on reserve mobilization during germination processes and seedling establishment presented a lot of variability due to the type of nanoparticles, sizes, forms, and doses. High concentrations of Fe3O4 NPs prevented the growth. Disorder is explained by a decrease in metabolite levels (such as amino acids and soluble sugar). According to the findings, Fe3O4 NPs2 had a greater favorable effect on seed germination and growth than Fe3O4 NPs1. It has been concluded that Fe3O4 NPs2 is not phytotoxic, and it may be possible to utilize them in the development of new agricultural products.

