

Introduction
Palynology has been revealed as one of the most prominent and prestigious fields for identifying and classifying mainly related taxa [1]. The term palynology comes from the Greek word “Palynein”, which is linked with the Palynomorphs study, which means dust [2]. Due to a wide range of pollen variations, they are well-defined and crucial in systematic research [3]. The palynology of medicinal plants was examined for the first time in Pakistan [4]. For this reason, taxonomists and researchers conduct a comprehensive analysis of many aspects of plant morphology to identify the correct name of the plant species [5]. Several researchers have carried out the palynology of Boraginaceae [6-10]. The diversity of species in phylogenetic and taxonomic systems was studied using pollen attributes [11, 12]. Pollen morphology is a significant method for resolving problematic taxonomic contests and has been used to categorize the taxa of Boraginaceae into tribes and subfamilies [13, 6]. The field of palynology is effective in the duplication of genes, generating cell toxins, and gene expression. For correct and proper identification and classification of angiosperms, various kinds of problems have been recognized using pollen morphology in other fields, including paleontology, plant taxonomy, and geology [14-16]. The diagnostic pollen characteristics of Boraginaceae are important in the taxonomy field, investigated by many researchers [6, 17].
LM and SEM provide enhanced and superior quality attributes of pollen because of their higher resolution power and create new terminologies in terms of pollen sculpturing pattern, pollen type, and ornamentation, which help in identification [1, 5, 18, 19]. SEM is also very useful for properly identifying different plant species using exine ornamentation [20, 21]. The palynological investigation of pollen was used to study the exact pollen morphology as well as the medicinal value of various plant species [22]. Since Erdtman’s work, pollen micromorphology has been a significant way for both identification and exact classification [23].
The Boraginaceae are found in diverse habitats, and collections of various taxa are located primarily in temperate regions worldwide, including about 130 genera and 2300 plant species [24], where Pakistan represented 32 genera with 135 plant species [6]. Additionally, the taxa in this family are also observed in tropical and subtropical zones of the world. Some of Boraginaceae’s diagnostic vegetative and floral characteristics include scorpioid cymose inflorescence, gynobasic style, and diverged ovary eventually developed into 4-nutlets, which could help perfect identification [6]. Additionally, the plant taxa of the Boraginaceae also have a considerable role in medicine and cosmetics [6, 25]. Various kinds of trichomes, which are epidermal attachments, are present on the leaves and stems of Boraginaceae, such as unicellular, multicellular, glandular, non-glandular, and acute. The presence of various types of trichomes can aid the taxonomic study of Boraginaceae. It is a complex field involving many different disciplines and tools that taxonomists use to categorize species into their appropriate categories. However, during the past 100 years, the tribal taxonomy of the Boraginaceae has evolved [26]. Modern taxonomy incorporates an assessment that considers significant morphological characters in addition to pollen when classifying plant species [1, 2, 4, 27]. Harmomegathy is an attractive adaptation in the pollen grains of Boraginaceae that helps them stay healthy in various environments. This includes folding pollen grains when they evaporate water, keeping them from drying out too much.
The taxa of the Borage family are usually europalynous and exhibit a diverse range of palynology, which makes the differences between various genera and species within the taxonomic group [6, 28]. Such variations in the shape of pollen grains and folding tricks help these plant taxa in wet and dry zones. Some tribes of the Boraginaceae family showed pollen that is heterocolpate, a type of pollen that is extremely rare in angiosperms with six to ten apertures; the small-sized, equatorial view is rectangular-elliptic, with or without narrowing at the equator; exine thickness is 0.5 to 1.0 pm; and psilate surface along grains outside of the colpus. Pollen grains vary considerably in morphology, resulting in a wide range of exine sculpturing, size, shape, and other characteristics [2, 3, 21, 29]. This study aims to provide novel information about the pollen attributes of Boraginaceae taxa while evaluating the systematic relevance of these pollen traits within the taxonomy domain. The examined pollen features prove valuable in both the identification and classification of Boraginaceae species, providing vital indicators for association with the taxonomic attributes specific to each species.
Materials and Methods
Plant Materials, Identification, and Deposition
Plant samples of Boraginaceae taxa were systematically collected through comprehensive field expeditions conducted in arid and semi-arid regions of Lakki Marwat, Dera Ismail Khan, Bannu, Karak, Kohat, Parachinar, Malakand, Sindh, and Baluchistan during the period from April to July 2023. The plants were collected, photographed, and brought into the laboratory for identification and microscopic study. The plant species were verified with those found in the Herbarium of Pakistan (ISL) using available published sources. The taxa were further verified with the help of The Plant List (www.theplantlist.org) and The World Flora. After authentic identification, the ethanol and mercuric chloride solution was used to poison these plant specimens. The newly collected poisonous plant specimens were shade-dried before placement and tagging on appropriate herbarium sheets [1, 2, 5, 6, 21]. The poisoned voucher specimens were delivered to the Herbarium of Pakistan (ISL), QAU Islamabad.
Investigation of Pollen Morphology Using Light Microscopy
Mature pollen grains were taken from the collected flowers and placed on a new, clean slide. With the help of the acetolysis method, the pollen grains have been prepared for light microscopy [30]. A small rod was employed to beat the pollen after it had been treated with acetic acid to make the pollen move out of the flower’s anthers. The debris was scraped using a needle, and the rest of the pollen on the slide was treated with glycerin jelly. It was made using the technique described by [1, 3, 21, 31]. The coverslips were placed over the slides, which were then studied under a light microscope (LM). The slides were marked with labels; the voucher number and name of the species were written down and placed upright in a wooden box. On each slide, the number of pollen grains was quantified. A microscope (MEIJI, Japan) was utilized for the micrometric analysis of pollens, and an Infinity 1-5C-MEL (Canada), armed with an LM LEICA DM 1000, was employed for micrographs. The following parameters were considered for morphometric studies: polar and equatorial diameter, length and width of colpi, exine thickness, and mesocolpium. Qualitative examination of pollen encompasses an assessment of its attributes, including its shape as indicated by the P/E ratio, dimensions, the pollen dispersion unit, and exine sculpturing. Using the IBM SPSS software, the results of morphometrics were aggregated to provide a statistical summary, encompassing the mean value, the range from minimum to maximum, and standard error [2, 4, 5].
Scanning Electron Microscopy as a Tool for the Investigation of Taxonomic Features
The techniques recommended by [21, 32] were used in preparing pollen grains for SEM analysis. We used scanning electron microscopy (SEM) to conduct an in-depth examination of the exine thickness, number of colpi, number of pores, and attractive coating. The pollens were acetolyzed and placed in 90% ethanol for SEM examination. Afterward, gold was affixed to a metallic rod pre-coated with palladium and then put together with metallic stubs. The photographs of pollen samples were captured using a scanning electron microscope (SEM) of the JEOL JSM5910 model present in the CRL of the Physics Department, University of Peshawar, Pakistan.
Statistical Analysis
In this research, various quantitative and qualitative micro-morphological features were investigated. To facilitate the analytical phase, we used SPSS 16.0 software to quantitatively compute essential parameters, such as mean, maximum, minimum, and standard error (SE) of any attribute about pollen characteristics [1-3, 5, 6]. The pollen shape was determined using the ratio of polar to equatorial diameter. Terminology was used to assess the size as well as the shape of pollen [33]. The statistical program XLSTAT version 2018 was used to evaluate the variance between seven variables for the PCA: polar diameter, equatorial diameter, P/E ratio, colpi length and breadth, exine thickness, and mesocolpium of the studied species.
P/E Ratio
The shape of pollen may be determined by applying the provided formula [34].
P/E = PA/ED×100
PA showed the polar axis, and ED showed the equatorial diameter of pollen.
Polar Fertility and Sterility Estimation
The number of viable and sterile pollens was assessed on each slide. Pollen that was damaged, broken, or improperly dyed was deemed sterile, whereas pollen that was effectively stained was assumed to be fertile.
The mathematical formula described by [35] was used to calculate pollen fertility and sterility percentages.
Fertility = F/F + S×100
Sterility = S/S + F×100s
Results
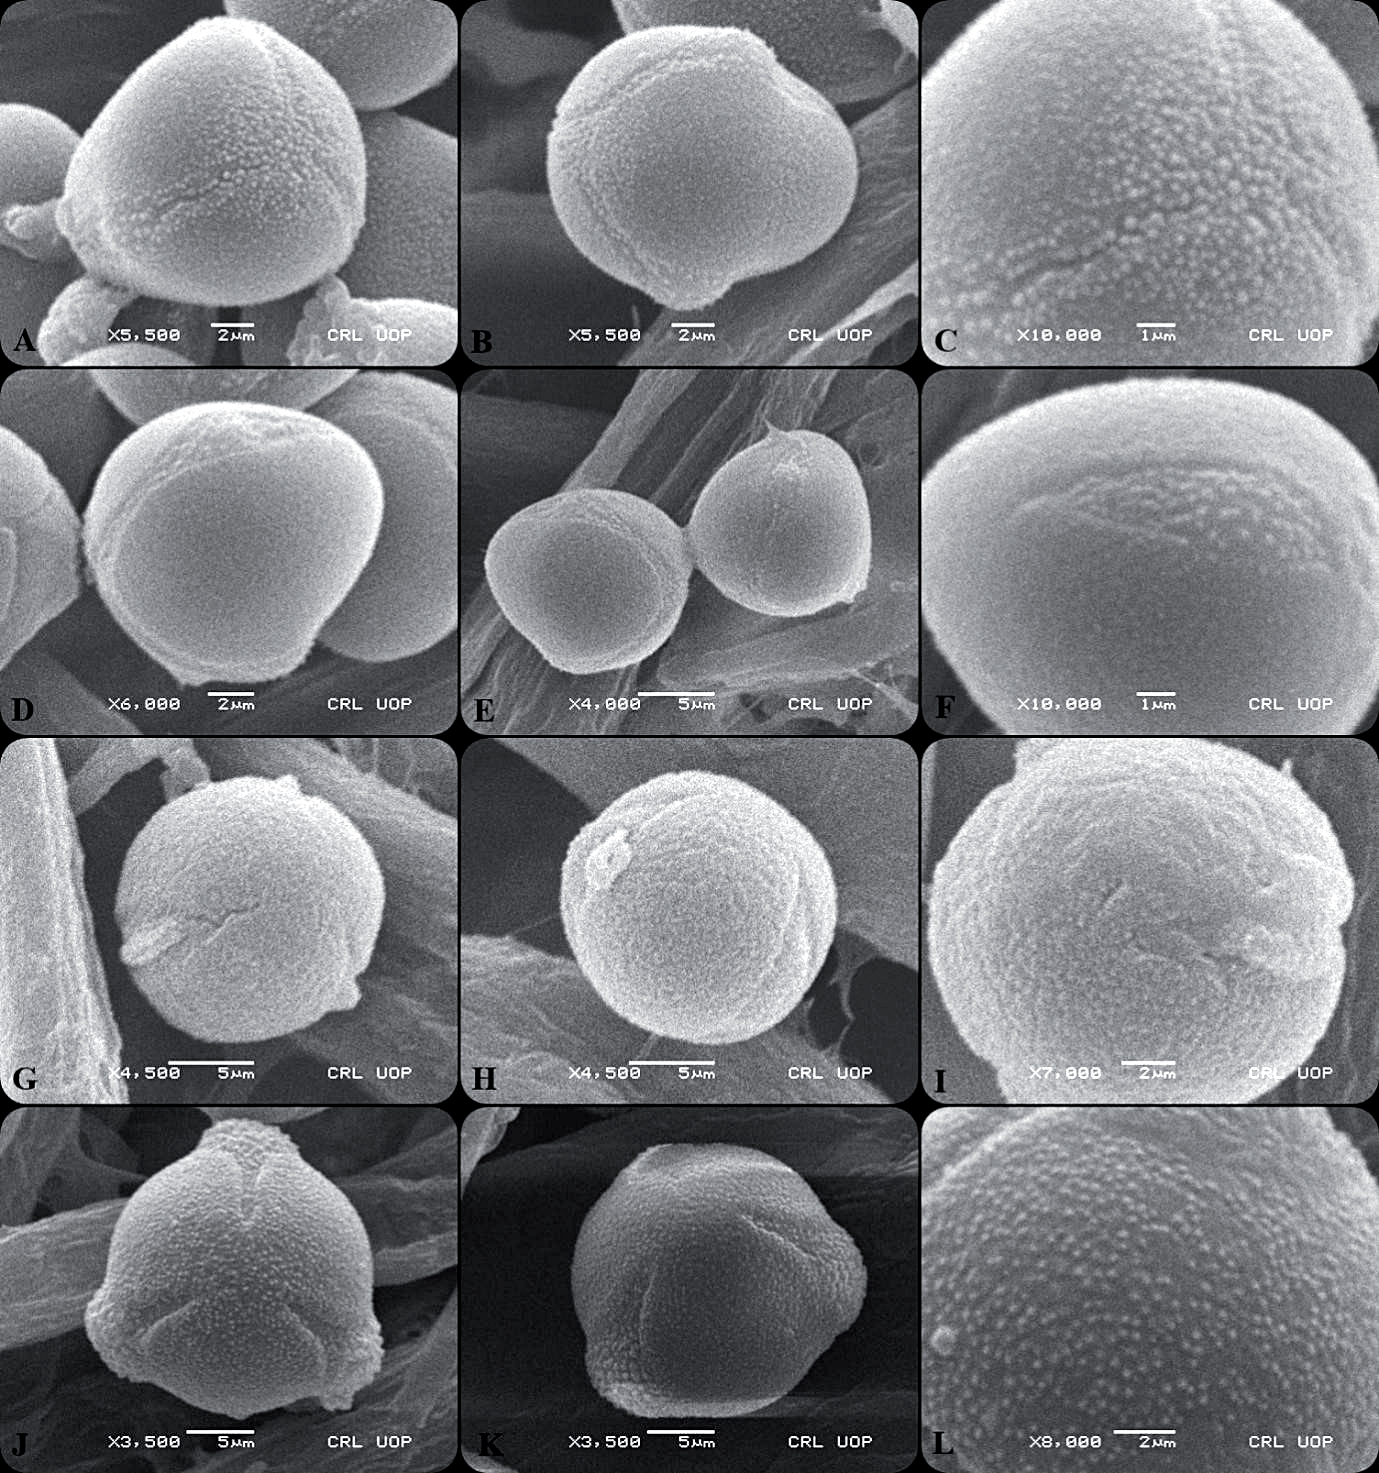
In the current research, LM was used to examine the palynomorphological aspects of 24 species of Boraginaceae. The exact identification among various species belonging to the same family or genus was achieved through careful analysis of the morphological attributes of pollen grains, including the shape, size, surface ornamentation, and existence of distinctive patterns and apertures. The morphological attributes of pollen are evaluated using the techniques of light microscopy and scanning electron microscopy and are properly compiled in quantitative and qualitative form as well. The investigation noted pollen morphological variations in the pollen form of the Boraginaceae family species. These morphological features must be present for the accurate identification of plants. The pollen grains of the species under research display monad as a morphological trait, showing shapes oblate, peroblate, suboblate, oblate-spheroidal, prolate, and perprolate. The pollen grains ranged from very small to medium-sized and showed polarity of both types, such as isopolar and heteropolar. Each investigated species exhibits a different aperture number and condition. Pollen surfaces include psilate, sub-psilate, echinate, foveolate, striate, and scabrate (Figs. 1-6).
Dispersal Unit and Size
The current study found that all pollen grains from the investigated taxa under examination exhibited a monad structure. Small-sized pollens were noticed in Anchusa arvensis, Arnebia benthamii, Arnebia decumbens, Buglossoides arvensis, Caccinia macranthera, Gastrocotyle hispida, Onosma bracteosa, Onosma dichroantha, Onosma hispida, and Onosma limitaneum. The medium-sized pollens were observed in Alkanna tinctoria, Arnebia grandiflora, Arnebia speciosa, Euploca strigosa, Heliotropium supinum, Nonea caspica, Nonea edgeworthii, and Trichodesma indicum. Pollen grains that are very small to medium-sized were recorded in Arnebia griffithii, Cynoglossum lanceolatum, Heliotropium bacciferum, Heliotropium curassavicum, and Heliotropium europaeum. The highest polar diameter among all the investigated taxa was recorded at 41.83±0.5 µm in Alkanna tinctoria, and the smallest was in Arnebia decumbens at 11.12±0.4 µm. The equatorial diameter was largest in Alkanna tinctoria, 45.66±0.7 µm, and the smallest was recorded in Cynoglossum lanceolatum, 9.66±0.2 µm. The maximum P/E ratio was observed in Arnebia hispidissima 1.4. The maximum length of the colpi was 3.75±0.3 µm, observed in Heliotropium supinum, while a conversely diminutive measurement of colpi length was found in Caccinia macranthera at 0.91±0.3µm. Similarly, the highest colpi width was observed in Euploca strigosa at 5.91±0.4 µm, whereas the lowest width of colpi was recorded at 1.12±0.1 µm in Caccinia macranthera. The highest exine thickness was recorded at 3.12±0.3 µm in Arnebia speciosa, while the lowest value was present at 0.95±0.1 µm in two species, including Buglossoides arvensis and Onosma hispida.
Shape and Polarity
The investigated species exhibit a wide range of variations in their shape, where the dominant shape was prolate to spheroidal, noticed in Buglossoides arvensis, Gastrocotyle hispida, Heliotropium bacciferum, Euploca strigosa, and Trichodesma indicum. The oblate shape was found in Anchusa arvensis, Arnebia grandiflora, and Caccinia macranthera. Suboblate pollens were observed in Arnebia benthamii, Arnebia griffithii, Heliotropium curassavicum, Heliotropium europaeum, and Heliotropium supinum. The subprolate shape was present in Onosma dichroantha and Onosma hispida. Similarly, the oblate-spheroidal shape was present in Alkanna tinctoria, Arnebia speciosa, Nonea edgeworthii, and Onosma bracteosa. Only Arnebia hispidissima and Onosma limitaneum possess the prolate shape. The perprolate shape was observed in a single examined species, Cynoglossum lanceolatum. They showed both types of polarity: isopolar and heteropolar.
Pollen Fertility and Sterility Percentage
The percentage of pollen fertility and sterility of the investigated species was determined. The highest percentage of pollen fertility was recorded in Onosma hispida (92.14%), whereas the lowest percentage was observed in Onosma limitaneum (56.82%). Onosma limitaneum (43.18%) was recorded as the highest sterility of pollen, while the lowest pollen sterility was observed in Onosma hispida (7.86%).
Pollen Types
The most prevalent pollen type among all the taxa under study was tricolporate, followed by tetracolporate, tetracolpate, pentacolpate, hexacolpate, hexacolporate, heterocolporate, and octacolporate. Tricolporate pollen was the distinguishing feature of Alkanna tinctoria, Anchusa arvensis, Caccinia macranthera, Onosma bracteosa, Onosma dichroantha, Onosma hispida, Onosma limitaneum, and Trichodesma indicum. The tetracolporate pollen was recorded in Arnebia benthamii, Arnebia decumbens, Arnebia grandiflora, Cynoglossum lanceolatum, Nonea caspica, and Nonea edgeworthii, tetracolpate in Arnebia griffithii, pentacolpate in Arnebia hispidissima, hexacolpate in Arnebia speciosa, hexacolporate in Buglossoides arvensis, Gastrocotyle hispida, and Heliotropium supinum, heterocolporate in Heliotropium bacciferum, Heliotropium curassavicum, and Heliotropium europaeum, and octacolporate pollen was observed only in Euploca strigosa.
Exine Ornamentation
The exine ornamentations of the taxa in Boraginaceae exhibit discernible variations in the ornamentation pattern of exine, such as reticulate, psilate, granulate, psilate-granulate, perforate, and psilate-perforate. The reticulate sculpturing was observed in Alkanna tinctoria, Anchusa arvensis, Arnebia benthamii, Gastrocotyle hispida, and Onosma bracteosa, psilate in Arnebia decumbens, Cynoglossum lanceolatum, granulate in Arnebia grandiflora, Arnebia griffithii, Arnebia hispidissima, Arnebia speciosa, Heliotropium bacciferum, Heliotropium curassavicum, Heliotropium europaeum, Euploca strigosa, Heliotropium supinum, Onosma dichroantha, Onosma hispida, Onosma limitaneum, and Trichodesma indicum, psilate-granulate in Buglossoides arvensis, perforate in Nonea caspica, and psilate-perforate in Nonea edgeworthii.
Discussion
In the present study, microscopic tools were used to find the latest information on the micromorphological attributes of the Boraginaceae across different geographic zones within Pakistan. According to [21, 36], the palynological characteristics were considered useful for classifying species and genera. The Boraginaceae family is europalynous and heterogeneous in terms of pollen features [5, 18]. A total of 24 species belonging to 11 distinct genera within the Boraginaceae family were systematically collected across various zones of Pakistan. Different pollen characters were studied for all the selected taxa. Studying pollen characteristics lets us determine the micro-morphological features that recognize similarities and dissimilarities among various species [37]. The pollen grains within this family are almost monad, very small in size, and show shapes such as oblate, suboblate, oblate-spheroidal, prolate, perprolate, subprolate, and prolate-spheroidal. They show both isopolar and heteropolar types of polarity [5, 21].
Fig. 1.
Scanning electron microscope photograph. A-C) Alkanna tinctoria. D-F) Anchusa arvensis. G-I) Arnebia benthamii. J-L) Arnebia decumbens.
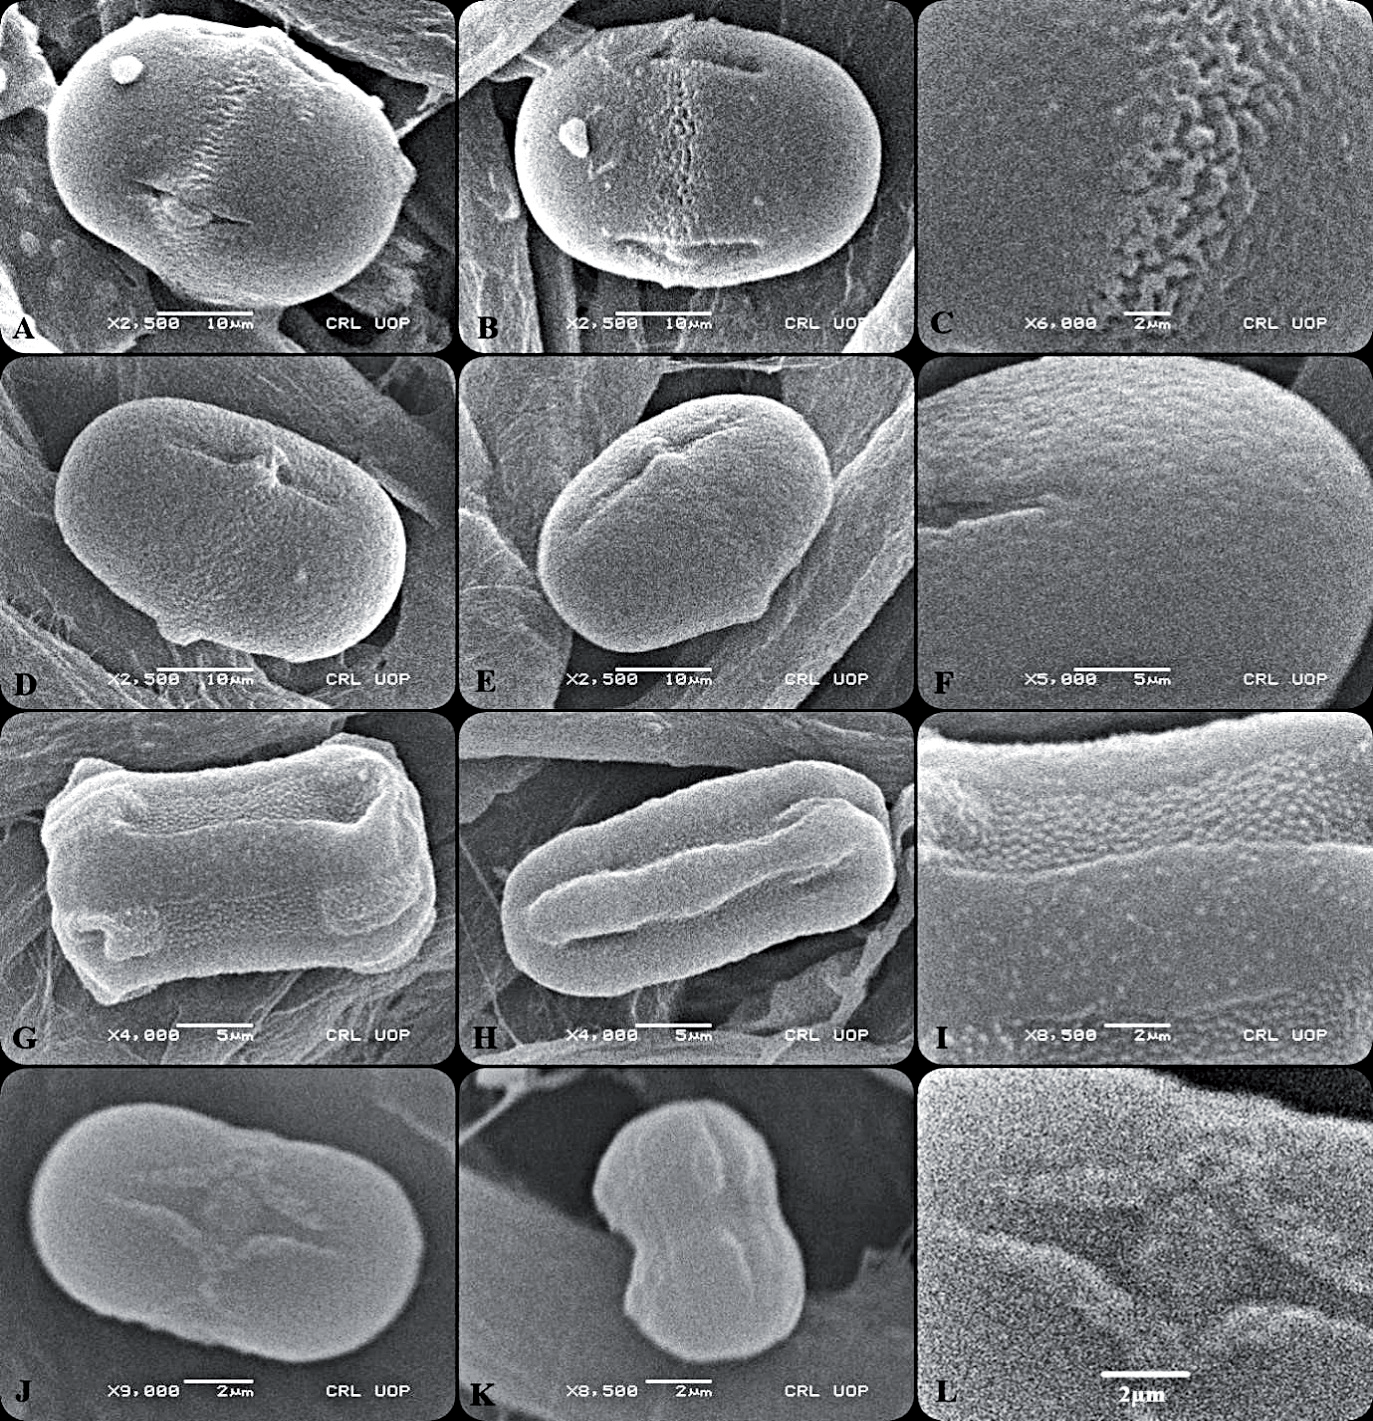
Alkanna tinctoria, Arnebia speciosa, Nonea
edgeworthii, and Onosma bracteosa show the same pollen shape as oblate-spheroidal, but they show variation in pollen size, as Alkanna tinctoria, Arnebia speciosa, and Nonea edgeworthii are medium-sized pollen, whereas small pollen grains were observed in Onosma bracteosa [21]. Anchusa arvensis shows a resemblance to Arnebia grandiflora and Caccinia macranthera in pollen shape as oblate, and they also have the same pollen size as small, except for Arnebia grandiflora having medium-sized pollen grains. Suboblate types of pollen were found in Arnebia benthamii, Arnebia griffithii, Heliotropium curassavicum, Heliotropium europaeum, and Heliotropium supinum. Still, they also found variation in their pollen size, as Arnebia griffithii, Heliotropium curassavicum, and Heliotropium europaeum were small to medium-sized pollen, whereas small and medium-sized pollen were observed in Arnebia benthamii and Heliotropium supinum, respectively. Arnebia hispidissima and Onosma limitaneum show similarities in both pollen shape (prolate) and size (small). Similarly, Buglossoides arvensis, Gastrocotyle hispida, Heliotropium bacciferum, Euploca strigosa, and Trichodesma indicum show their shape as prolate-spheroidal, which is the dominant shape of the investigated species. They are dissimilar in pollen size; however, Buglossoides arvensis and Gastrocotyle hispida have small-sized pollens, whereas Heliotropium bacciferum has small to medium-sized pollens, and medium-sized pollens were found in Euploca strigosa and Trichodesma indicum. Pollen grains of different species of Onosma investigated in this study were small, heteropolar, tricolporate, colpi apex acute, prolate-oblate spheroidal-shaped, and exine ornamentations were granulated, while pollen grains in the previous study were heteropolar, subprolate, and tricolporate and had a rounded polar outline, which looks similar to our results [5, 17].
Fig. 2.
Scanning electron microscope photograph. A-C) Arnebia grandiflora. D-F) Arnebia griffithii. G-I) Arnebia hispidissima. J-L) Arnebia speciosa.
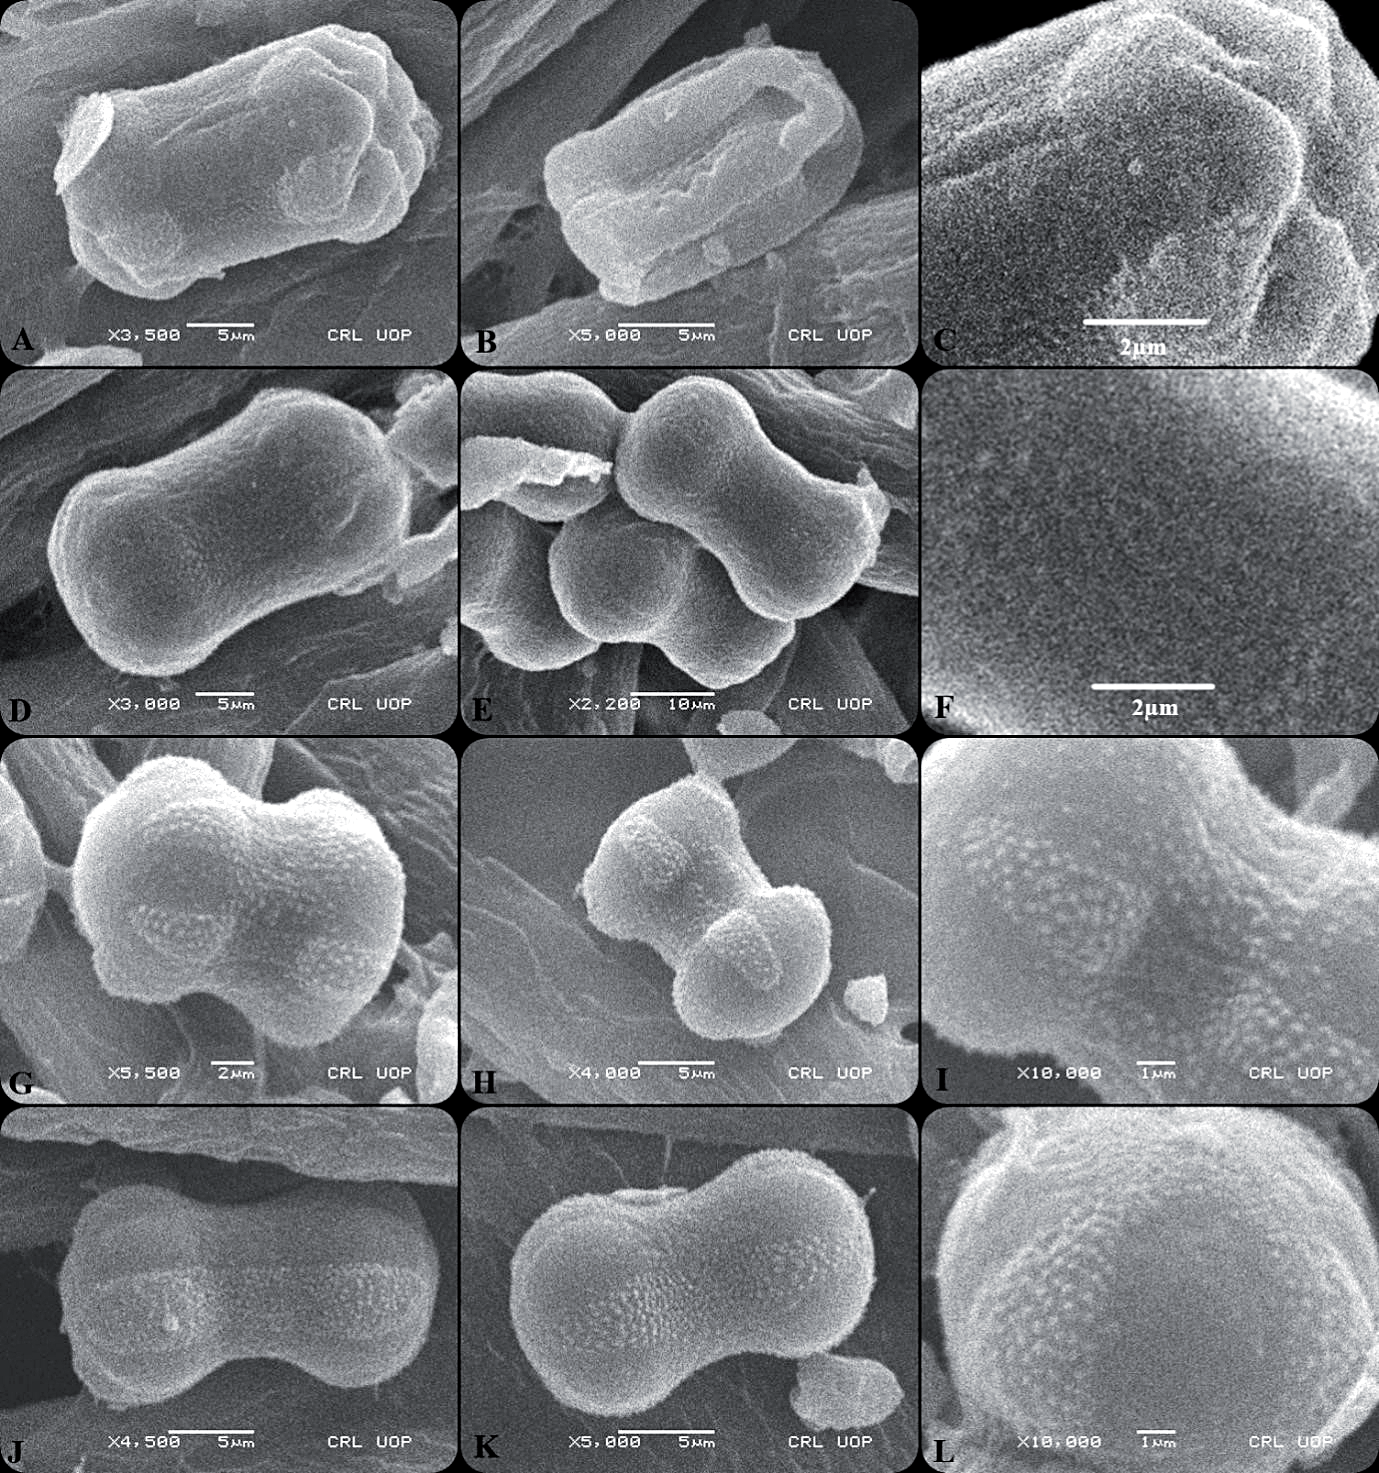
Many taxonomic keys have been introduced to differentiate across plant taxa and speed up the determination of species based on palynology. The pollen shape, type, and exine ornamentation of Alkanna tinctoria were oblate-spheroidal, tricolporate, and reticulate, respectively. The shape, type, and aperture of Anchusa arvensis were reported to be prolate, tricolporate, and zonoaperturate, which were comparable to our findings [9]. However, the exine sculpturing varied greatly in both studies; they noticed a fossulate-foveolate exine sculpturing pattern, while in our study, it was reticulate. The characteristic feature of zonoaperturate pollen in Arnebia benthamii was parallel to our results. Unlike the investigations of [38], which represented prolate to perprolate, 4-6 colporate pollen type, and micro-echinate, our study disclosed the type of pollen, exine pattern, and shape of pollen that were tetracolporate, reticulate, and suboblate. Pollen shape diverged greatly in both types of analysis, with suboblate in our findings and prolate in theirs.
Fig. 3.
Scanning electron microscope photograph. A-C) Buglossoides arvensis. D-F) Caccinia macranthera. G-I) Cynoglossum lanceolatum. J-L) Gastrocotyle hispida.
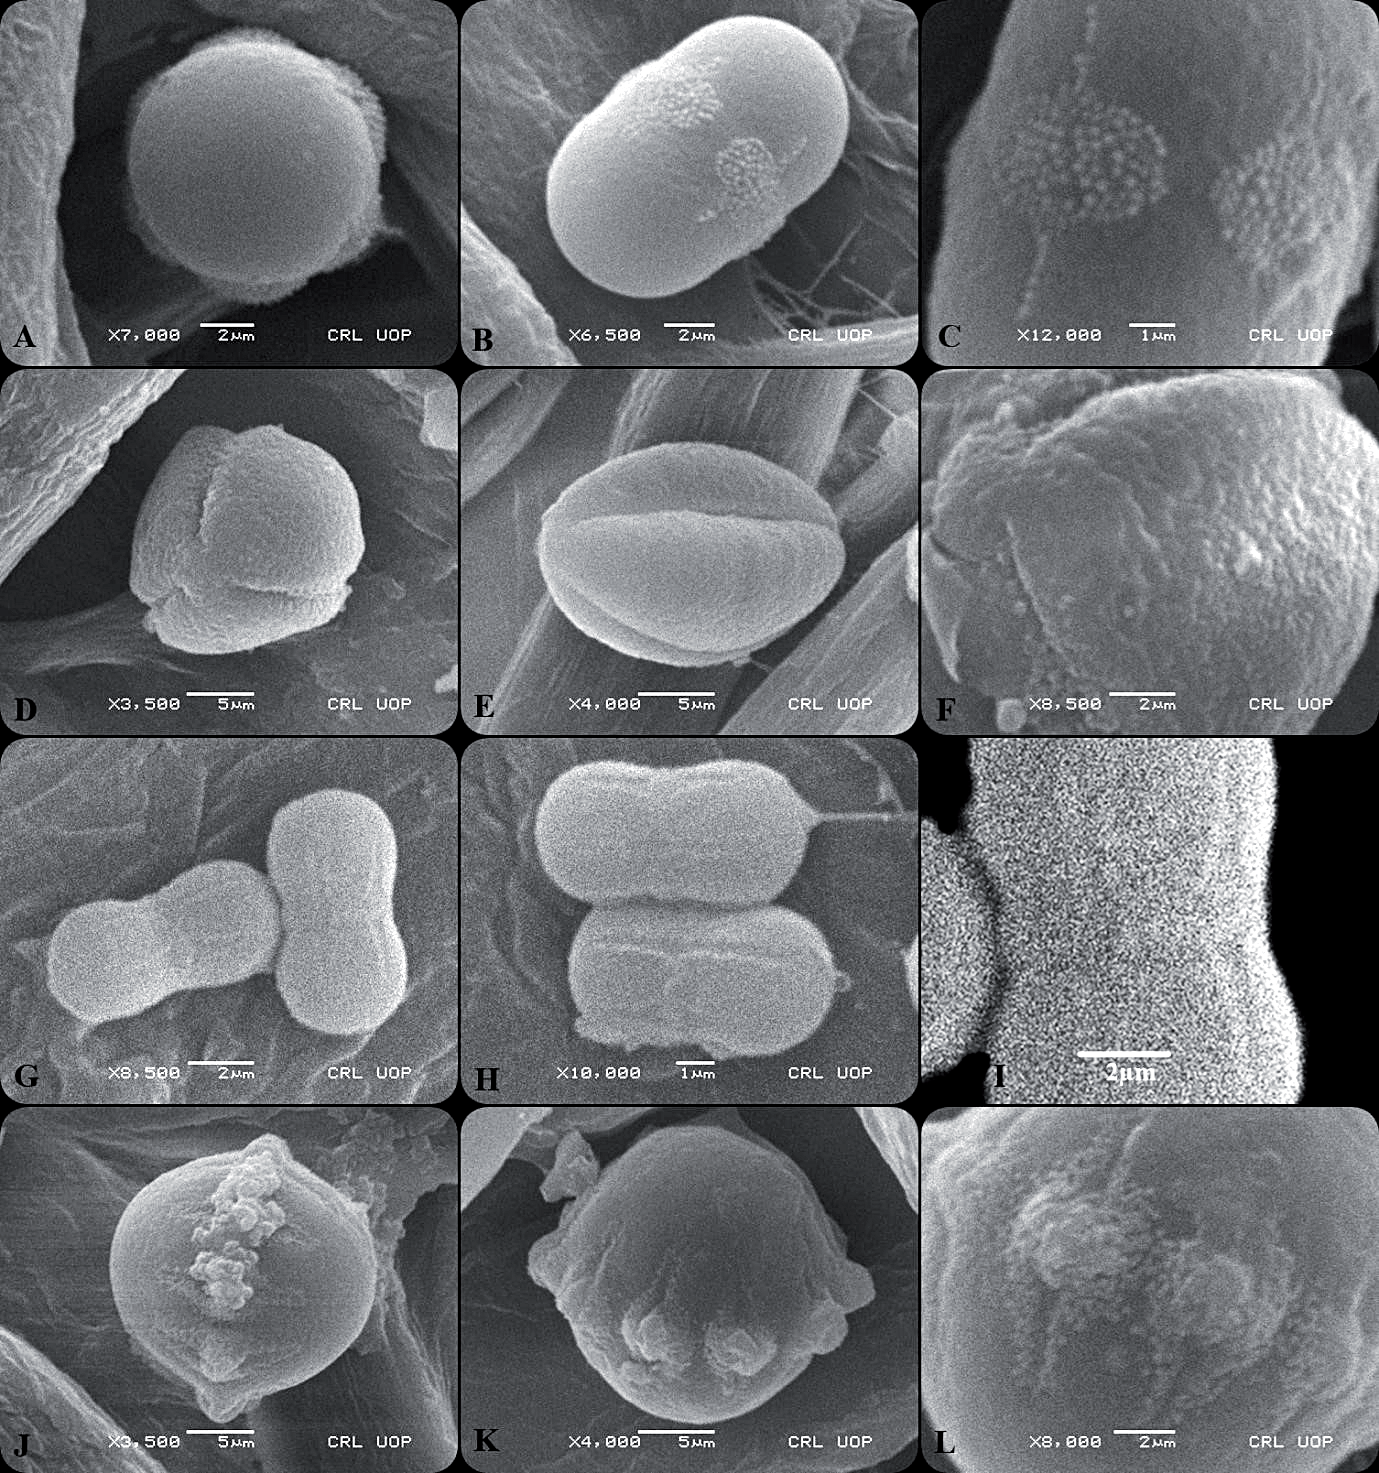
The prolate pollen shape of Arnebia grandiflora was indicated by [5, 6], while granulate, oblate, and tetracolporate pollen were revealed in our findings. The investigated pollen of Arnebia griffithii shows similarities with the described pollen morphology by [39], representing an echinate sculpturing, 4-syncolpate pollen type, and prolate shape, whereas in investigations of [20], the pollen shape and exine ornamentation were found to be peroblate and verrucate pollen patterns. Variations in pollen shape and exine ornamentation are described as suboblate and granulate. According to [40], the pollen attributes of Arnebia hispidissima were isopolar pollen, prolate, 6-colpate, and found to be prolate, isopolar, 6-colpate, and generally wider and dipped near the equator. [41] found parallel results described as colpate, stephanoaperturate, and isopolar pollen in Arnebia hispidissima, while representing variations in pollen shape and surface sculpturing as prolate and granulate. According to [20], the pollen morphology of Arnebia hispidissima was found to be isopolar, peroblate in shape, 5-colpate pollen type, and micro-echinate in surface. The shape, pollen type, polarity, and exine pattern of Arnebia speciosa were disclosed by our investigations, showing oblate-spheroidal, 6-colpate, isopolar, and granulate ornamentation. Similarly, 6-colporate pollen, isopolar, zonoaperturate, and psilate-granulate pollen surface of Buglossoides arvensis were observed by [42], which are in line with our study. However, the pollen shape of Buglossoides arvensis shows variation as prolate-spheroidal. Our results revealed that the pollen morphology of Caccinia macranthera, described as oblate-shaped, 3-colporate in type, isopolar, and reticulate exine sculpturing. The shape, pollen type, and exine surface of Cynoglossum lanceolatum were described as perprolate, 4-colporate, and psilate pollen, elucidated by our study. As also reported by [28], the spheroidal, isopolar, colporate, and perforate pollen are the characteristic features of Gastrocotyle hispida. However, the pollen shapes were examined to be prolate in our study. Furthermore, the number of colpi in hexacolporate differs, which indicates pentacolporate and octacolporate, respectively.
Fig. 4.
Scanning electron microscope photograph. A-C) Heliotropium curassavicum. D-F) Heliotropium europaeum. G-I) Euploca strigose. J-L) Heliotropium supinum.
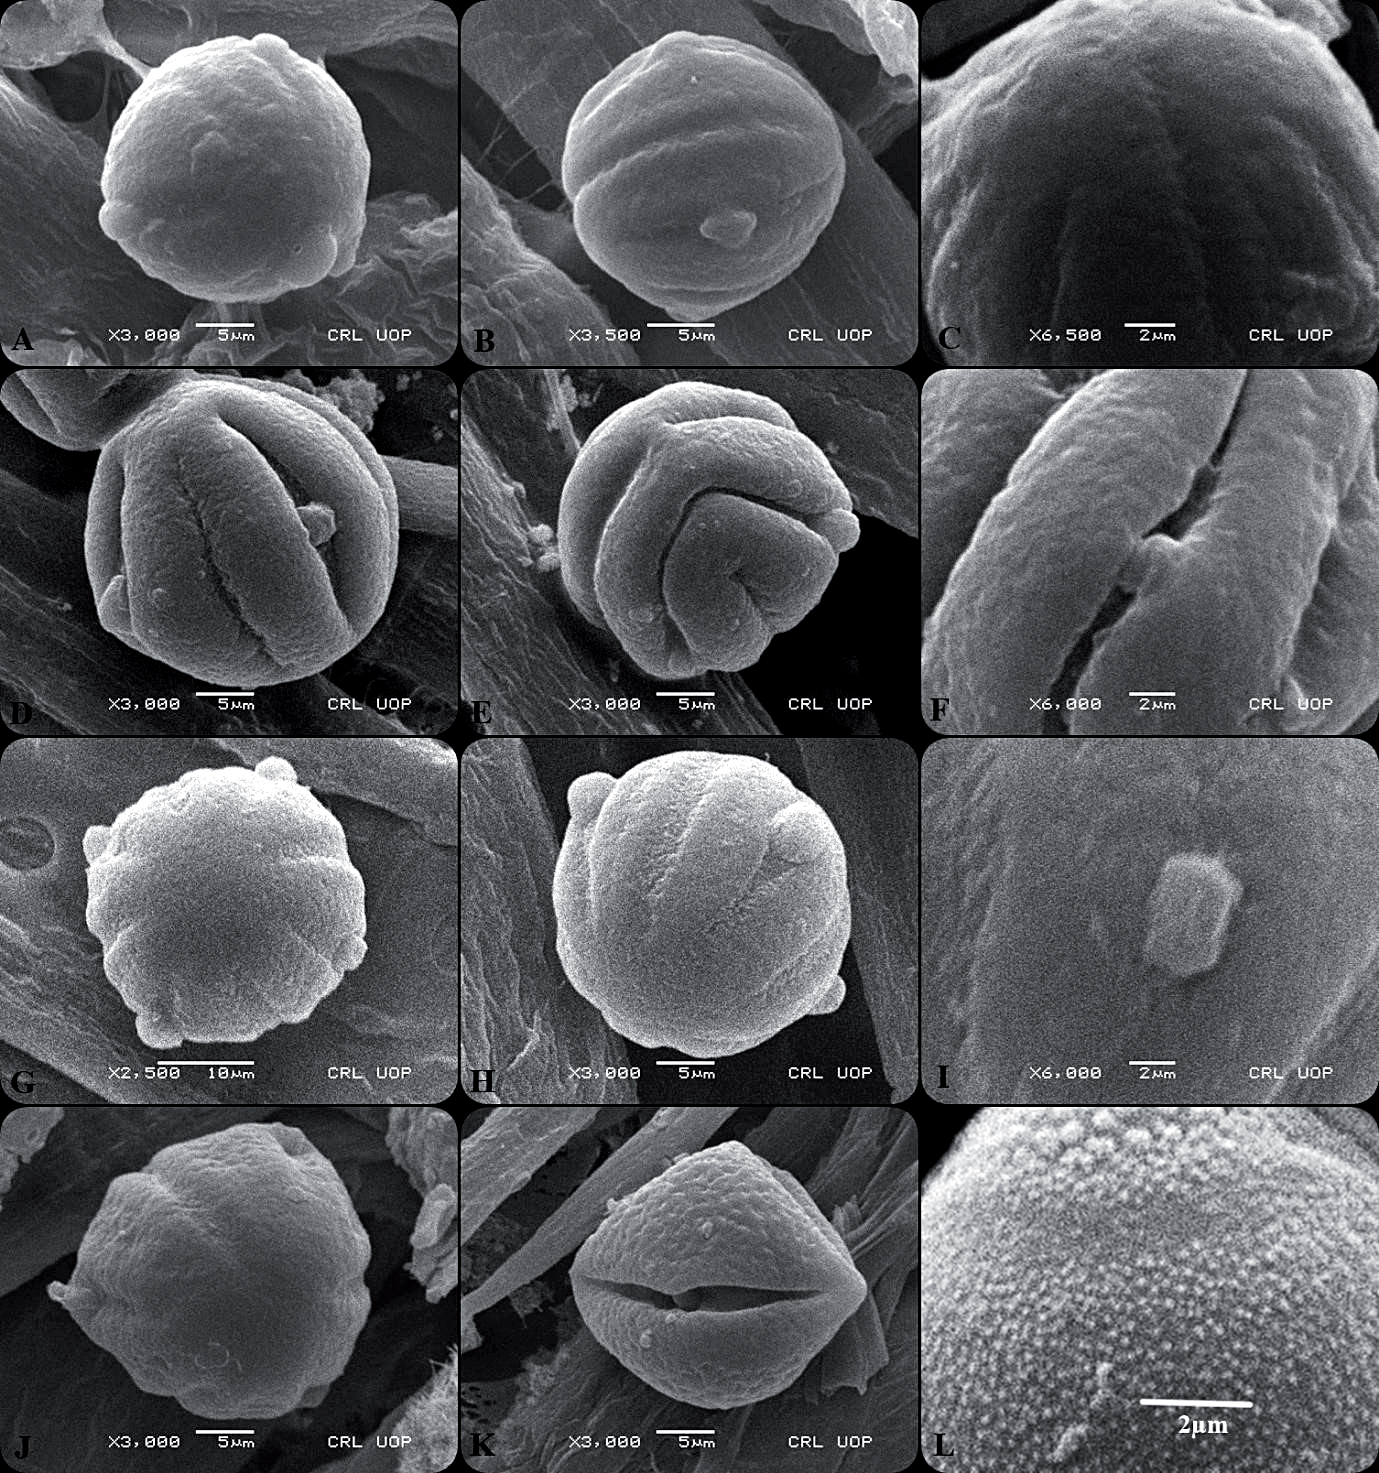
The pollen grains of Heliotropium bacciferum are prolate or prolate to spheroidal with an 8-heterocolporate, a correspondence that is the same as the outcomes obtained in our study [43]. The pollen of Heliotropium bacciferum was described as prolate, isopolar, regulate, and pseudocolpate by [43]. Except for exine ornamentation, which is referred to as granulate, we obtained findings that were mostly comparable to those characters provided by [44]. Prolate and 6-heterocolpate pollen were reported in Heliotropium curassavicum by [28]. According to [20], the shape, polarity, pollen type, and exine pattern of Heliotropium curassavicum were observed as suboblate, isopolar, heterocolporate, and verrucate, while within the purview of our findings, the shape and exine ornamentation of pollen in Heliotropium curassavicum underwent a subtle change, manifesting as suboblate and granulate. The reported pollen of Heliotropium europaeum is prolate and 6-heterocolporate; however, the same results were revised to reveal prolate, 3-colpate, isopolar, pseudocolpate, and scabrate [45]. The present study’s aperture type and pollen polarity are comparable to those of [39], but other characteristics, such as pollen shape along with 4-stephanocolporate, 4-pseudocolpate, and granulate, show variations. Pollen of Euploca strigosa was recorded by [46], indicating a prolate, isopolar, 6-8 heterocolporate pollen. Still, our results revealed a variance in shape, aperture, and exine surface characterized by prolate-spheroidal, 8-heterocolporate, and granulate. Similarly, the pollen of Heliotropium supinum described by [46] presented prolate-spheroidal, isopolar, and 6-heterocolporate pollen, whereas our study disclosed the variations in shape and exine surface characterized by suboblate and granulate, respectively. Our study of the pollen of Nonea caspica exhibits variations in palynology with [46], indicating a prolate and reticulate surface, but our study disclosed the shape and exine surface as suboblate and perforate. Polarity, pollen type, and aperture show similarities in both investigations, described as isopolar, tetracolpate, and zonoaperturate. The oblate-spheroidal, isopolar, tetracolporate, and psilate-perforate pollen were the characteristic features of Nonea edgeworthii. Our investigations disclosed the pollen morphology of Onosma bracteosa, characterized by oblate-spheroidal, isopolar, tricolporate, and reticulate pollen. According to [46], the shape, polarity, type, and exine surface of Onosma dichroantha and Onosma hispida were suboblate, heteropolar, tricolporate, sub-psilate, and foveolate, but in our study, pollen shows variations only in shape and exine surface, described as sub-prolate and granulate in both species. Similarly, [46] described the pollen features of Onosma limitaneum as spheroidal, heteropolar, tricolporate, and scabrate, but our study shows variations only in shape and exine sculpturing reported as prolate and granulate. The pollen results were the same in both investigations; [46] described it as prolate-spheroidal, isopolar, tricolporate, and scabrate, but in our study, variations were found only in the exine surface as granulate.
Fig. 5.
Scanning electron microscope photograph. A-C) Heliotropium bacciferum. D-F) Nonea capsica. G-I) Nonea edgeworthii. J-L) Onosma bracteosa.
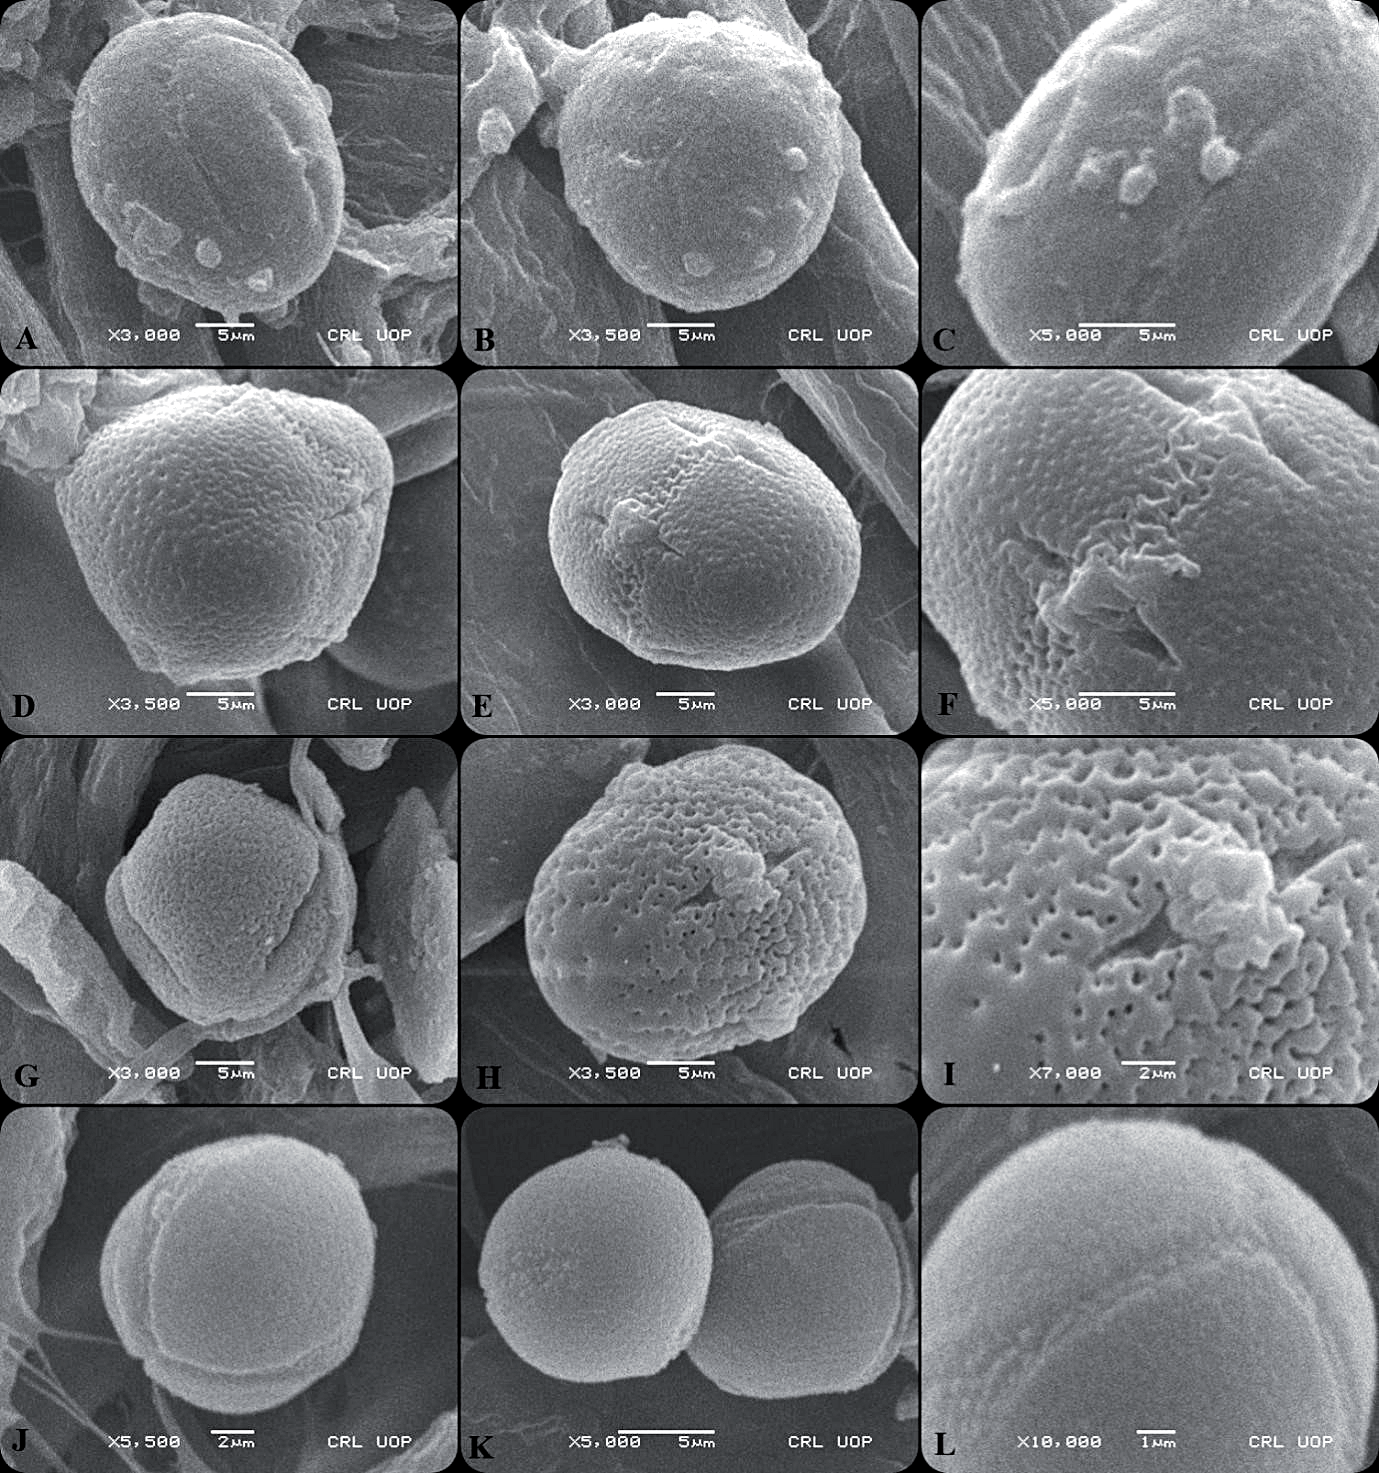
Fig. 6.
Scanning electron microscope photograph. A-C) Onosma dichroantha. D-F) Onosma hispida. G-I) Onosma limitaneum. J-L) Trichodesma indicum.
Furthermore, in aeropalynology, mellisopalynology, and geopalynology, the study of SEM and LM, even though their taxa are known, is of utmost benefit for identifying pollen formulas [1, 2, 4, 6]. The palynologists may find it helpful to use LM and SEM to accurately and swiftly identify plant species to create a global atlas of the Boraginaceae [5]. Further studies employing the worldwide taxa would help to reach more definitive conclusions.
Conclusions
In the present study, the pollen morphology of Boraginaceae was considered a vital component for facilitating the delineation of many different species. The study provides detailed knowledge of the taxonomic significance of the family’s closely related species and genera for the first time from Pakistan. The reported species showed variations in shape, size, and exine thickness, whereas prolate to spheroidal shapes were abundantly noticed in many species of the selected family. It was found that pollen morphometric and morphological features varied substantially. We also examined the most efficacious diagnostic features of Boraginaceae pollen and where these attributes may be employed in conjunction with other morphological features to delineate boundaries of species for comparative studies in the future. In the systematics of higher plants, the morphological characteristics of pollen were regarded as an important taxonomic tool. The research’s objective is to increase our understanding of a species’ morphology, which will aid in taxonomic research and, ultimately, the conservation of species in Pakistan.

