

Introduction
Moss is among the oldest nonvascular vegetation [1] and the most widely distributed plants across the planet [2]. Because of the high adaptability of moss to highly acidic and nutrient-deprived habitats [1], and its positive role in restoring and conserving degraded lands [3, 4], moss has seen increasing attention.
Most of the previous works concentrated on the distribution of mosses and their relationship with the environment [5]. Few works analyzed the impact of shading on moss, hindering our understanding and response to the impacts of future global changes. Shade is a passive means of relieving stresses by lowering heat and increasing available resources by increasing soil water. For most mosses, lowered light is not a stress since they tolerate or desire low light contexts [6, 7]. On the one hand, increasing global shade causes shifts from mosses to vascular vegetation [8]. On the other hand, moss growers introduce extensive shading treatment to reduce water loss and the impacts of increasing drought. Although many efforts provided assistance in understanding the ecological impact of moss from the perspectives of soil physicochemical attributes, plant productivity, and microorganisms, the influence of shading on soil attributes, moss traits, and moss-related microbiomes is poorly understood.
Studies have reported the effects of mosses on soil physicochemical attributes. The presence of moss significantly alters many attributes of the soil, especially electrical conductivity, and pH [9]. Moss releases hydrogen ions to acidify the soils or releases phenolics [1], thus changing soil pH. Their morphological and architectural properties and cell traits exhibit a high capacity for water storage and retention, can conserve soils [2], and reduce runoff [10] and water loss [11]. Moss thus increases soil moisture [12]. Some studies found that moss changes the soil organic matter density [12] and has positive effects on all soil nutrients [13, 14]. For example, moss increases soil organic carbon, total nitrogen, and available nitrogen concentrations [3], and converts unavailable potassium to available potassium [14]. Moreover, moss activates aluminum and iron oxides in the soil, thereby promoting the increase in mineral-bound organic carbon [1]. Besides, the capillary action of mosses in absorbing water can minimize the losses of soil organic matter, nitrogen, and phosphorus [14, 15]. However, others confirmed that moss maintains the contents of most fundamental nutrients at constant levels, whereas it shows minimal effects on soil macronutrients, such as the contents of soil phosphorus and potassium [16]. This discrepancy suggests the necessity of additional study.
Inconsistent conclusions remain exist regarding the effect of shading on moss traits. Some studies found that species often exhibit a maximum number of branches in fairly high-light contexts; however, higher radiation can expedite moss dehydration, consequently reducing growth [17]. Others showed the positive effect of shade on the yields of mosses [7, 18, 19]. Some degree of shading increases the cover, density, and productivity of mosses [7]. This discrepancy suggests the necessity of additional study. Furthermore, carbon, nitrogen, phosphorus, potassium, iron, and aluminum are the basis of plant physiology, growth, reproduction, structure, and functioning [20, 21]. Despite the significant roles the moss traits (i.e., the carbon, nitrogen, phosphorus, potassium, aluminum, and iron contents of moss) play in moss growth, photosynthesis, and environmental adaptability [20], the effect of shading on the moss traits is still not fully understood.
Like vascular plants [22], mosses host diverse microbiomes that have a significant and essential effect on host phenotype, environment adaptability, nutrient acquisition, productivity, and reproduction [1, 23-26]. Since the microbial community of mosses is hyper-sensitive to their physical environments, even when planted in almost homogenous environments [27], we speculate that the shading would restructure moss-related microbiomes. Furthermore, many previous studies have shown the diversity and composition of soil- or moss-related microbiomes [25, 28-30], their roles in the development of moss, and the biotechnological capability of microbiomes [31]; however, despite the important role moss epiphytic microbiomes play in moss adaptability [25, 28], how the shading reshapes moss epiphytic microbiome, and how moss epiphytic microbiomes link to moss traits remain unclear, especially for the bacterial and fungal communities on mosses’ phyllosphere and rhizoplane. Moreover, it remains unknown whether the shading changes the phyllosphere and rhizoplane microbial community composition, function, and network.
Therefore, in this study, we manipulated one-year-shading and non-shading treatments on artificially cultivated moss in the fields to determine the impacts of one-year-shading on the soil physical and chemical attributes, moss leaf and root traits, and bacterial and fungal communities on mosses’ phyllosphere and rhizoplane on the subtropical plateau of SW China, and to identify the biological drivers of moss trait. The following hypotheses (H) were tested: (a) one year-shading would change the phyllosphere and rhizoplane microbial community composition, function, and network (H1); (b) rhizoplane microbial community shows a more tightly relationship with the moss trait than phyllosphere microbial community does (H2).
Material and Methods
Study Area, Design, and Sample Collection
The study area (25°50′N – 26°10′N, 107°30′E – 107°50′E, 1412 m above sea level) was in a 100 mu common garden in Dushan county of Guizhou, SW China. This area is a subtropical monsoon humid region with an annual temperature of 13.9 °C and an annual precipitation of 1570 mm. Gleyed paddy soils cover this area.
Between late May and early June 2024, five sites under the treatments of shading and non-shading (i.e., five 1 m × 2 m plots) were established in short-term (one year) shading and non-shading areas, respectively. The shade was achieved by setting up shading nets, which can block 85% of the sunlight. First, in the 1m× 1 m subplot, 500 g fresh moss green part (leaves) and the yellow part (pseudo roots) were collected separately in sterile bags, stored under ice bags, and sent to Yangling Xinhua Ecological Technology Co., Ltd (Yangling, China) for testing the bacterial and fungal communities attached to the moss surface (i.e., phyllosphere and rhizoplane). To avoid cross-contamination, separate ring knives and sterile gloves were employed [32]. In the adjacent 1m × 1m subplot, the green part (leaves) and yellow part (pseudo roots) of all mosses were collected in sterile bags, killed at 105 ℃ and dried at 65 ℃ to constant weight, crushed by a grinder, sieved through a 2mm sieve, and used to determine plant traits. Three soil cores were collected using ring knives at each site. One was used to determine soil bulk density and soil porosity [32], while the other two were used to determine soil water holding capacity. Ca. 1kg 0-5 cm soil was collected for the assay of soil physicochemical attributes.
Assay of Soil Physicochemical Attributes and Moss Traits
This part was performed by Yangling Xinhua Ecological Technology Co., Ltd (China). Briefly, pH was tested using a pH meter [33]. Soil bulk density, total porosity, capillary porosity, and non-capillary porosity were tested [34] using an oven at 105 °C and an electronic balance (Shanghai Baiyinghengqi Corporation, China). Soil organic carbon content was tested using an elemental analyzer, available nitrogen content was analyzed by the alkali diffusion approach [35], available phosphorus content was tested using the sodium bicarbonate extraction-molybdenum antimony anti-colorimetric method [36], available potassium content was tested by the flare photometer method [32], available aluminum content was determined by the Hac-NaAc extraction and UV spectrophotometer and available iron content was determined by an atomic absorption spectrophotometer. Moss carbon content was tested using the potassium dichromate concentrated sulfuric acid external heating method [37], moss nitrogen content was determined using the H2SO4-H2O2 digestion and indigo phenol blue colorimetric method, moss phosphorus content was determined using the HNO3-HClO4 digestion method, moss potassium content was tested using the H2SO4-H2O2 digestion and flame photometry method, moss aluminum content was determined using the Nitric acid-perchloric acid digestion method, and moss iron content was determined using HNO3-HClO4 digestion method.
DNA (Deoxyribonucleic acid) Extraction, Amplicon Sequencing and Bioinformatics Analysis
This part was carried out by Novogene Biotech. Co., Ltd (CN). The method is available in supplementary documents. DNA isolation kits were applied to extract DNA. 16S rRNA and ITS genes of distinct regions (16SV3- V4 and ITS1-5F) were amplified. DADA2 (Divisive Amplicon Denoising Algorithm 2) was used to denoise [Version (Quantitative Insights Into Microbial Ecology) QIIME2-202202] for obtaining Amplicon Sequence Variants (ASVs). The bacteria and fungi were taxonomically named through QIIME2 with Silva and Unite Databases, respectively. The Chao1, Pielou evenness, Simpson, and Good coverage were calculated using QIIME2. To compare the differences between treatments, principal coordinate analysis was performed using “ade4” package and “ggplot2” package in R (v4.0.3). LEfSe (linear discriminant analysis effect size) was used to identify the indicators with linear discriminant analysis (LDA) scores ≥4 and statistically significant differences (p < 0.05) among treatments [35]. PICRUSt2 (Phylogenetic Investigation of Communities by Reconstruction of Unobserved States, V2.3.0) and FunGuild were applied to annotate the bacterial and fungal community’s functions. A bar chart and heat map with clusters were used to display the relative abundance through the “ggplot2” package and the “pheatmap” function. The network was established using the “igraph” package with removing the connections with Spearman correlation coefficient < 0.6 and connections with node abundance less than 0.005%. The raw data on bacterial (Accession number: SAMN43039897— SAMN43039878) and fungal (Accession number: SAMN43039877—SAMN43039858) microbiomes were uploaded to the National Center for Biotechnology Information (NCBI) in the name of PRJNA1144507.
Statistical Analysis
Wilcoxon test or Kruskal-Wallis test was applied to test the significance of difference [32] in the soil physicochemical attributes, moss traits, and microbial community diversity. To explore the relationships between moss traits and microbial properties, Pearson correlation analysis was applied using the “psych” and “igraph” packages in R v3.6.1. p < 0.05 suggests significant.
Results and Discussion
Shading Marginally Altered Soil Physicochemical Properties but Significantly Reduced Moss Root Aluminum
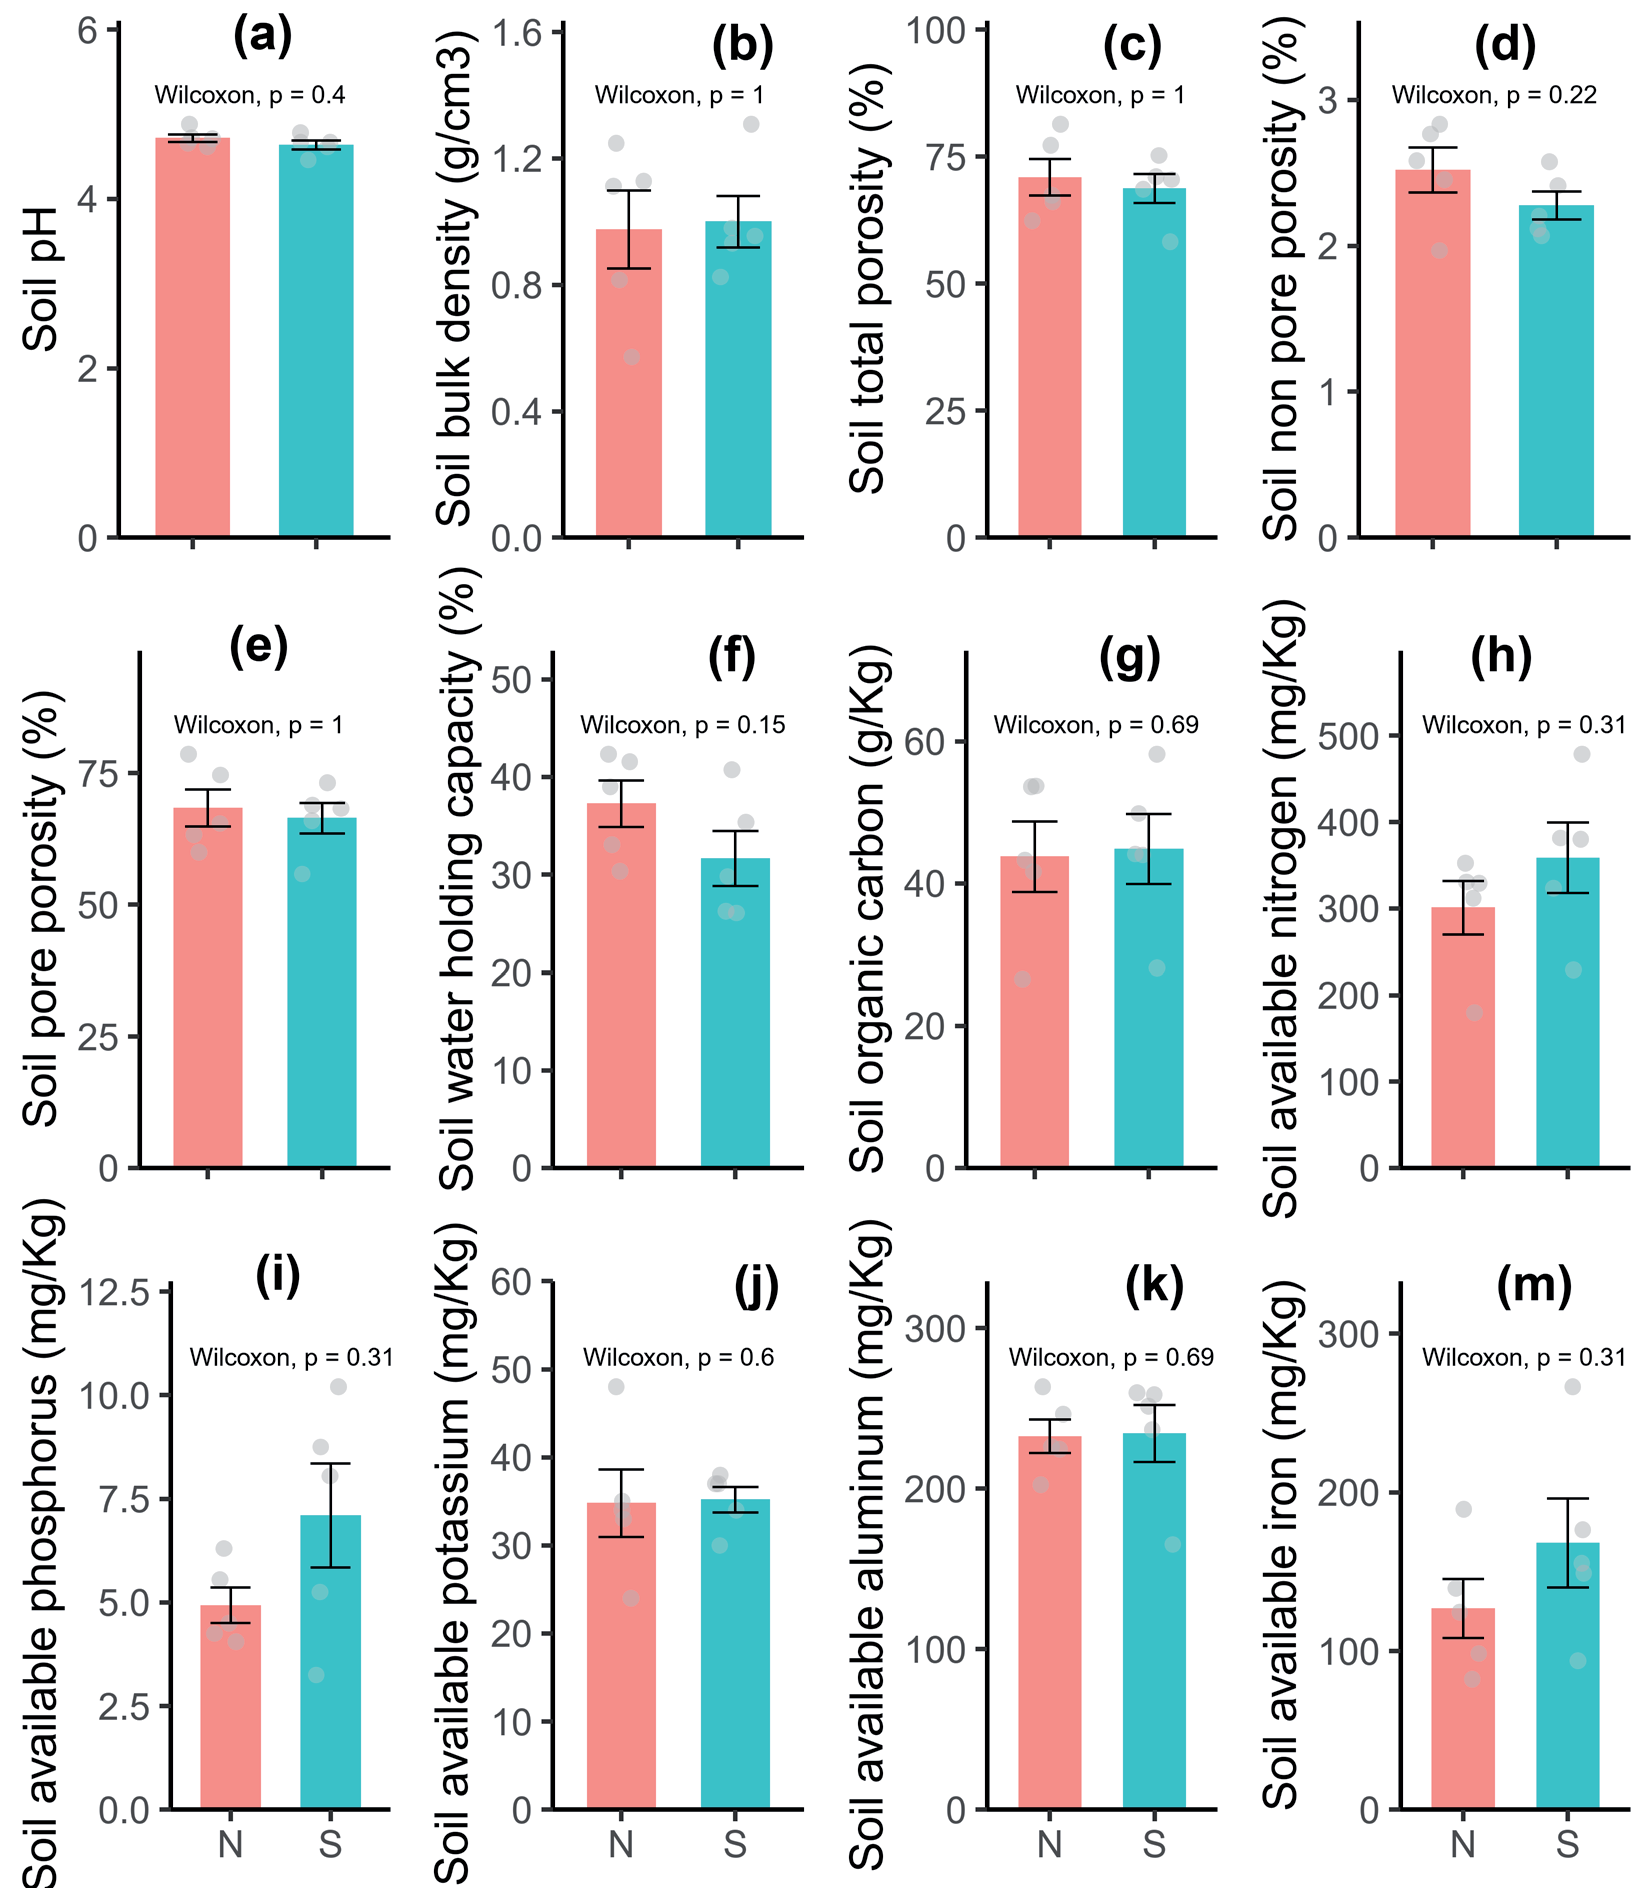
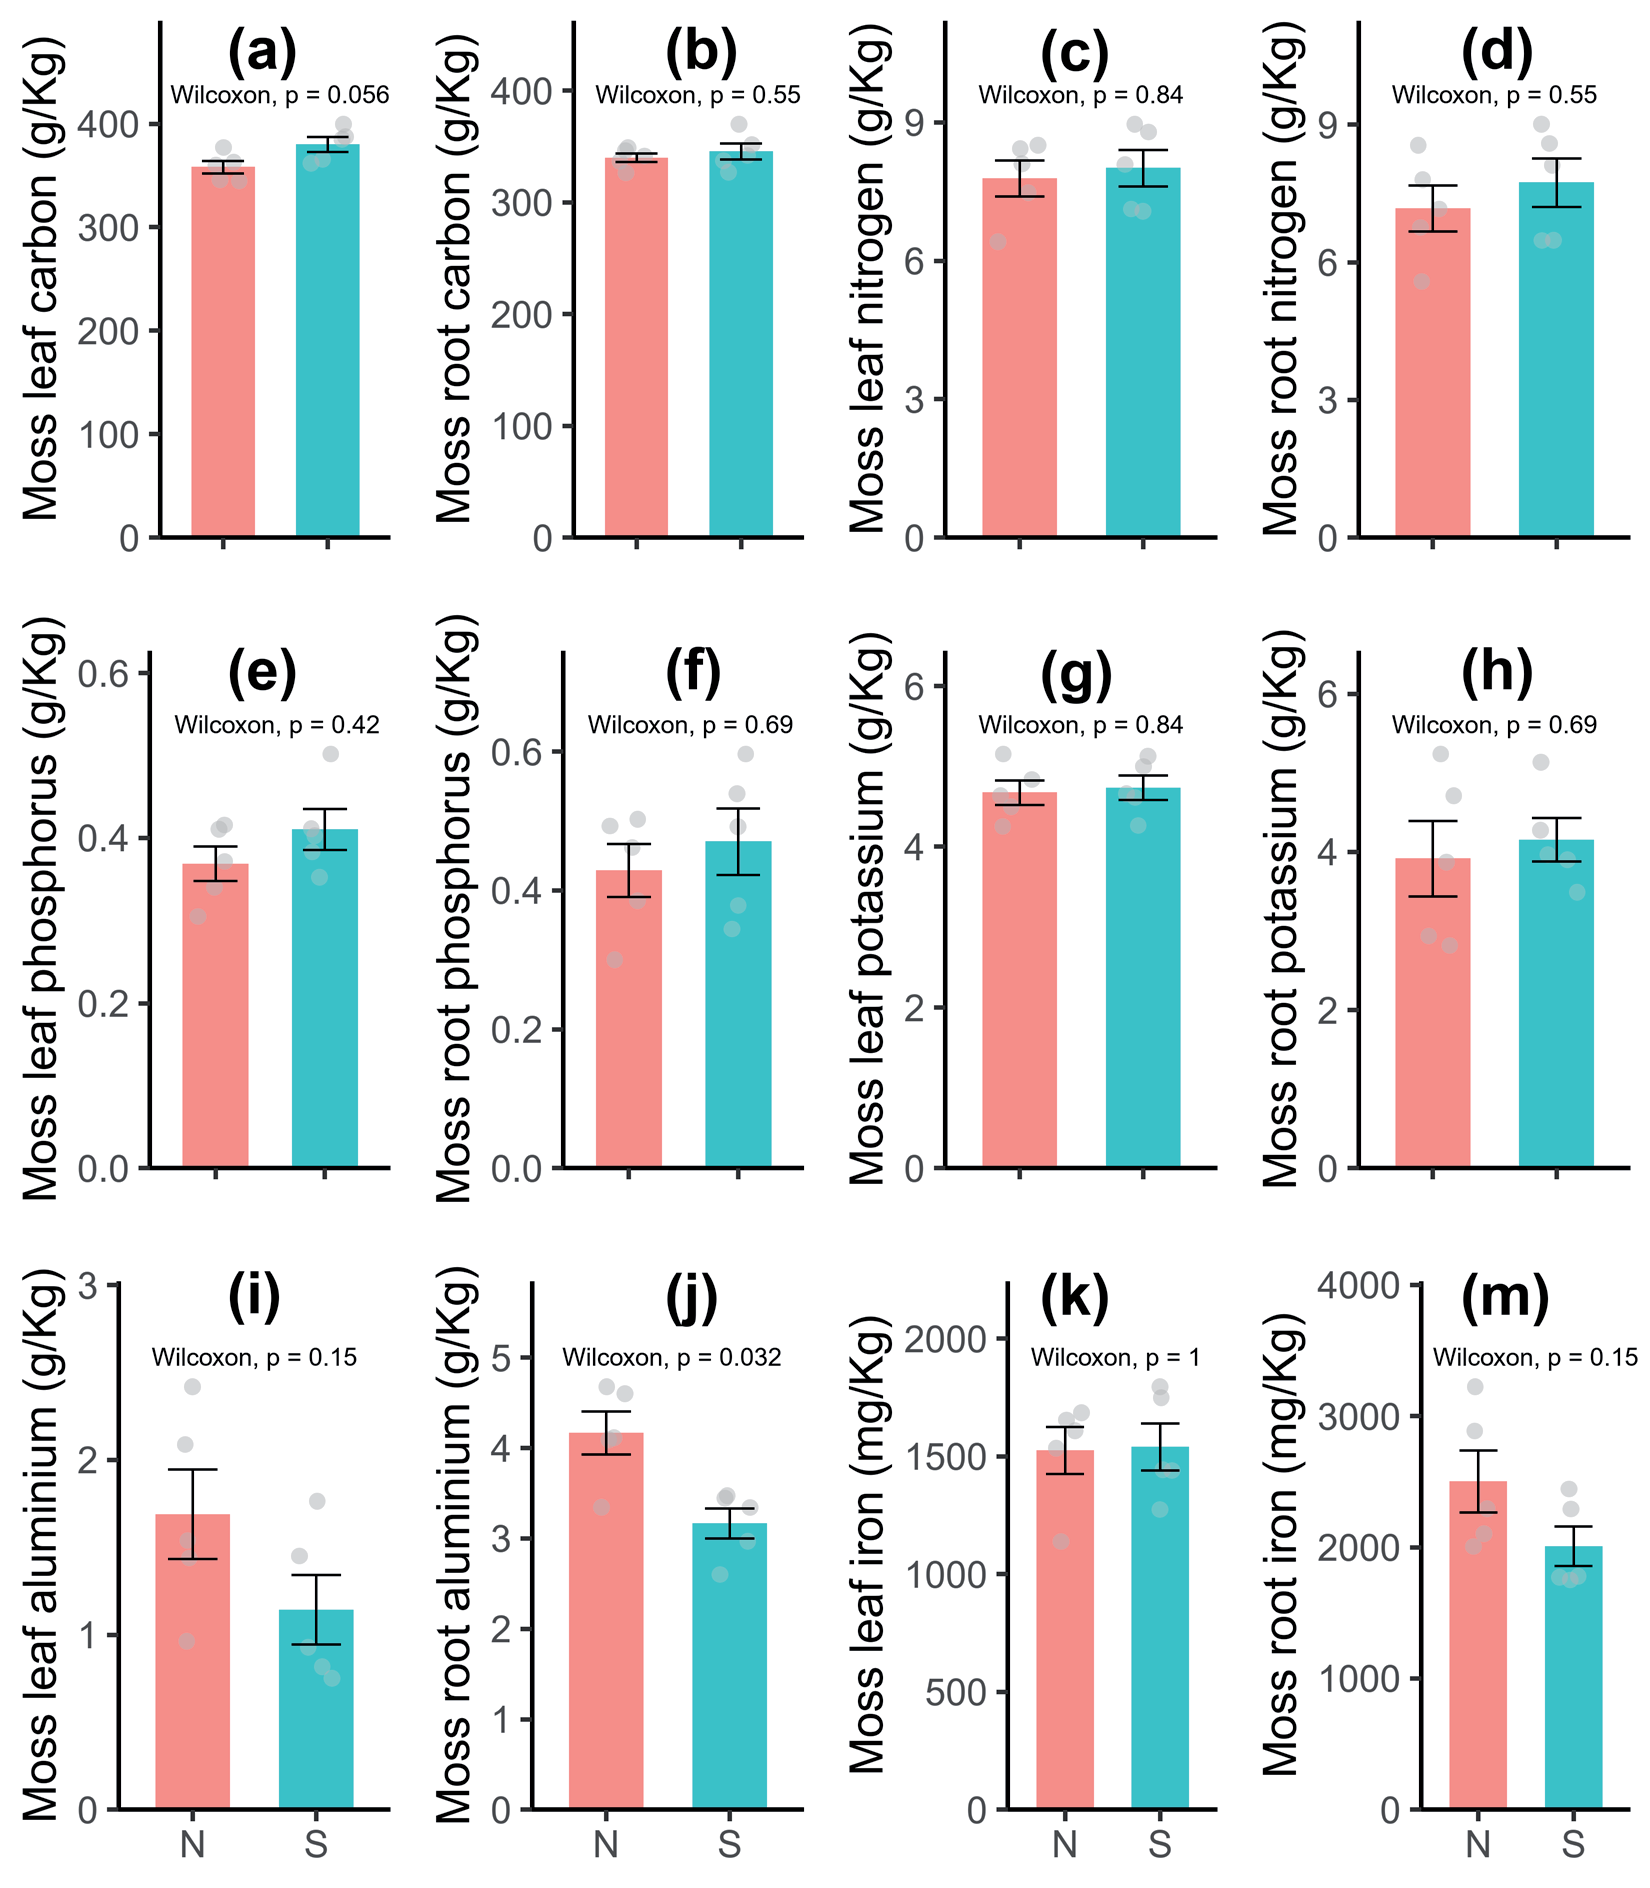
Shading treatment slightly changed the soil's physical and chemical properties (Wilcoxon test, p = 0.15-1, Fig. 1). The shading reduced soil and water loss [38], this might increase the soil organic carbon [3] (Fig. 1g). The shading increased nitrogen mineralization and nitrification rate and increased inorganic nitrogen [39]; this might increase soil available nitrogen [3] (Fig. 1h). Moss can release H+ to acidify soils (Wang et al. 2024), convert unavailable potassium to available potassium [14], and activate soil aluminum and iron oxides [1]. The shading might enhance this effect, thus increasing soil-available potassium (Fig. 1j), soil-available aluminum (Fig. 1k), and soil-available iron (Fig. 1m). Our evidence supported that the slightly positive effect of shading on soil chemical properties, although this needs further study. Nevertheless, further research is still needed on the mechanism by which shading decreases soil total porosity, soil non-pore porosity, soil pore porosity, and soil water holding capacity, and increases soil bulk density. Consistent with previous findings, shading increased the carbon and nitrogen content of dry mass [40] (Fig. 2a-d).
Compared with the non-shading, the shading did not significantly change the moss leaf carbon, moss root carbon, moss leaf nitrogen, moss root nitrogen, moss leaf phosphorus, moss root phosphorus, moss leaf potassium, moss root potassium, moss leaf aluminum, moss leaf iron, and moss root iron (Wilcoxon test, p = 0.056-1), however, shading significantly reduced the moss root aluminum content (Wilcoxon test, p = 0.032). Many studies have confirmed that aluminum in acidic soils has toxic effects on plants [41] and is a predominant cause restricting plant productivity in acidic soil [42]. The increase in soil available aluminum (Fig. 1k) might threaten the growth of moss; however, the shading marginally reduced the moss leaf aluminum content (Fig. 2i) and significantly reduced root aluminum content (Fig. 2j), implying that moss had strong adaptability to soil aluminum.
Shading Restructures Epiphytic Microbial Community
All good coverage was > 99.7% (Fig. S1), indicating an overall good sampling and sequencing depth [35, 43]. The chao1 (p = 0 – 0.0003), pielou evenness (p = 0 – 0.0003), Simpson (p = 0 – 0.0003) of rhizoplane bacterial community and the chao1 (p = 0.0003 – 0.0125) of rhizoplane fungal community were significantly higher than those of phyllosphere community (Fig. 3, Table S1). Although the shading increased the Chao1, Pielou evenness, Simpson of phyllosphere bacterial and fungal community and decreased the rhizoplane fungal community, compared with the non-shading, these changes were found to be insignificant (p = 0.2640 – 0.9208). In a word, the shading did not significantly change the phyllosphere and rhizoplane microbial community diversity. This result is similar to the effect of shading on the diversity of grass rhizosphere bacteria [44].
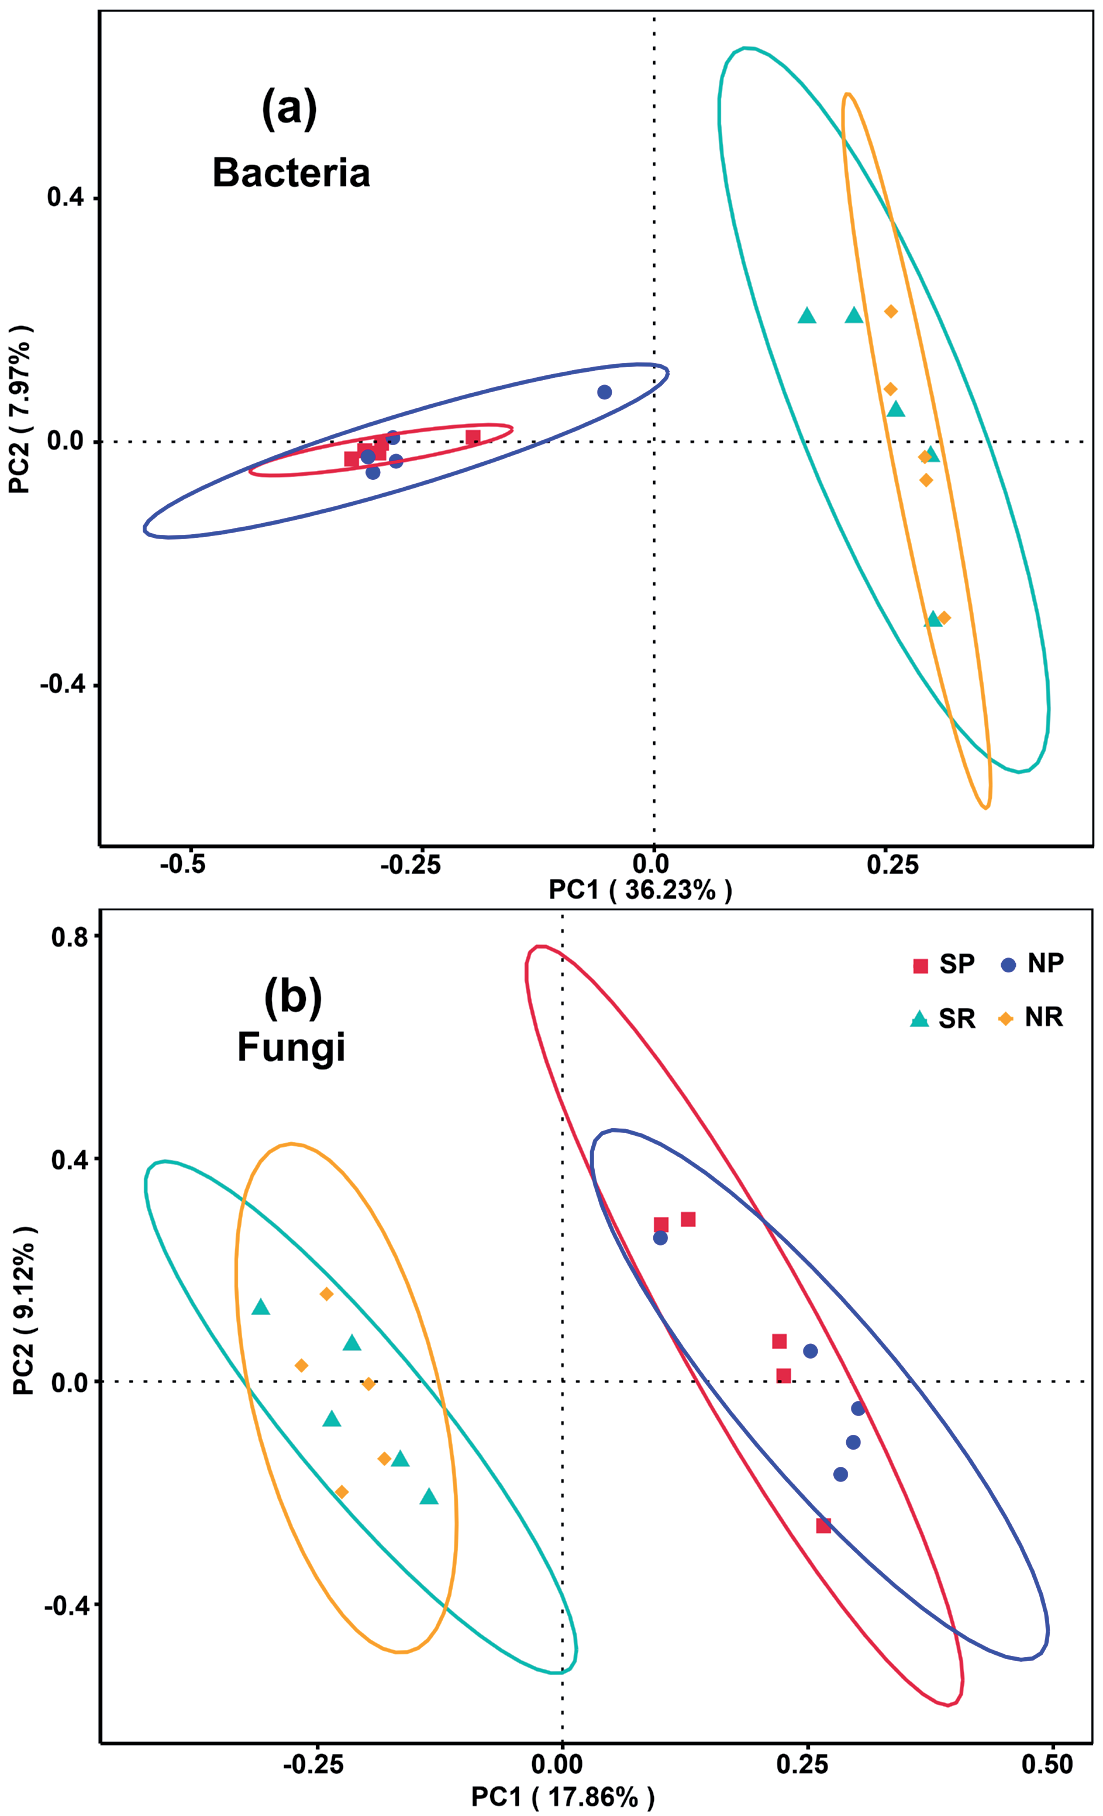
Overall, principal co-ordinates analysis (Fig. 4) suggested that there was a clear separation between the phyllosphere and rhizoplane microbial community composition, but there was no separation between microbial community composition under shading treatment and non-shading treatment, regardless of the phyllosphere or rhizoplane microbial community composition. At the phylum level, the bar chart showed that the shading increased the relative abundance of phyllosphere Proteobacteria, Acidobacteriota, Verrucomicrobiota, Bacteroidota, the relative abundance of rhizoplane Firmicutes, Verrucomicrobiota, Chloroflexi, the relative abundance of rhizoplane Ascomycota, and the relative abundance of phyllosphere Basidiomycota; however, the shading decreased the relative abundance of phyllosphere Firmicutes, Actinobacteriota, the relative abundance of rhizoplane Cyanobacteria, Proteobacteria, the relative abundance of phyllosphere Ascomycota, and the relative abundance of rhizoplane Glomeromycota. Previous studies showed that moss-related bacterial communities are dominated by the phyla Proteobacteria and Actinobacteria [25, 26, 28, 45, 46]. In this study, this situation was only found in the rhizoplane communities of moss, the phyla Proteobacteria and Cyanobacteria, rather than the phyla Proteobacteria and Actinobacteria dominated the phyllosphere bacterial communities of moss. Cyanobacteria, as epiphytes of mosses, are the dominant nitrogen-fixing organisms [47]; however, additional works are needed to test the effect of these differences on moss. Moreover, consistent with the previous findings [48, 49], the phyla Ascomycota and Glomeromycota dominated the phyllosphere and rhizoplane fungal communities of moss (Fig. 5c). Previous studies suggested that host phylogeny has a strong effect on the related microbiome and that niches also play key roles if the hosts are phylogenetically more similar [25, 46]. The present work showed a more important role of the moss compartment niche in structuring the moss epiphytic microbial community. Besides, this study provided more information than before, showing that the shading changed the relative abundance of the bacterial and fungal-dominated phyla (Fig. 5a, c).
Fig. 3.
The boxplot showing the effect of shading on the phyllosphere and rhizoplane bacterial (a-c) and fungal (d-f) community diversity. SP, moss phyllosphere under shading treatment; NP, moss phyllosphere under non-shading treatment; SR, moss rhizoplane under shading treatment; NR, moss rhizoplane under non-shading treatment; *, Kruskal-Wallis test p < 0.05; **, Kruskal-Wallis test p < 0.01; ***, Kruskal-Wallis test p < 0.001; non-significant (Kruskal-Wallis test p > 0.05) differences were not shown.
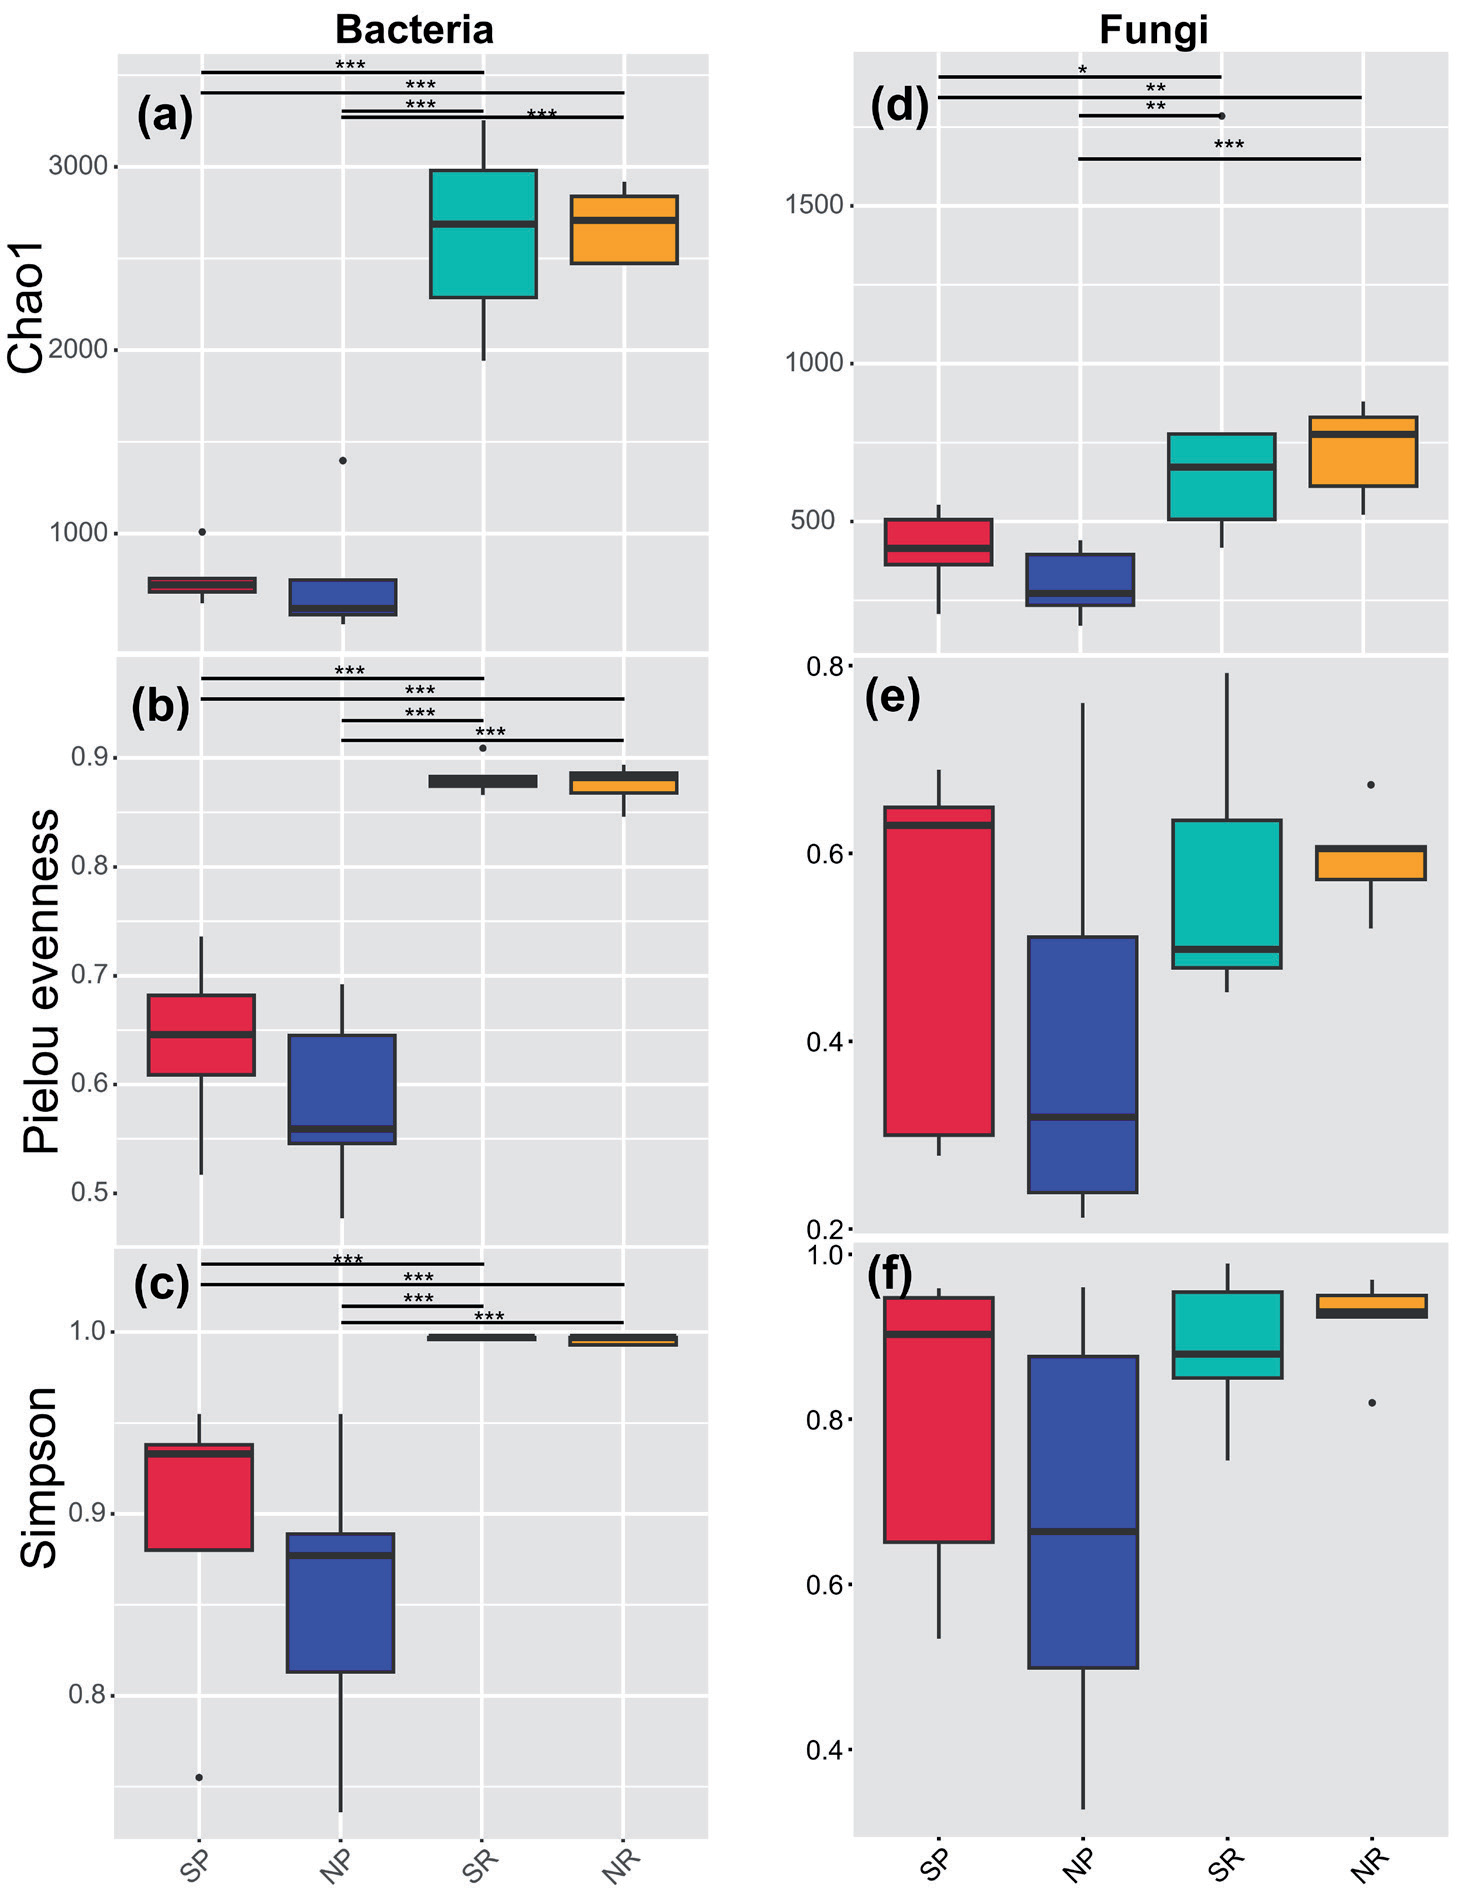
Fig. 4.
Principal coordinates analysis (PCoA) showing the effect of shading on the phyllosphere and rhizoplane microbial community composition. SP, moss phyllosphere under shading treatment; NP, moss phyllosphere under non-shading treatment; SR, moss rhizoplane under shading treatment; NR, moss rhizoplane under non-shading treatment.
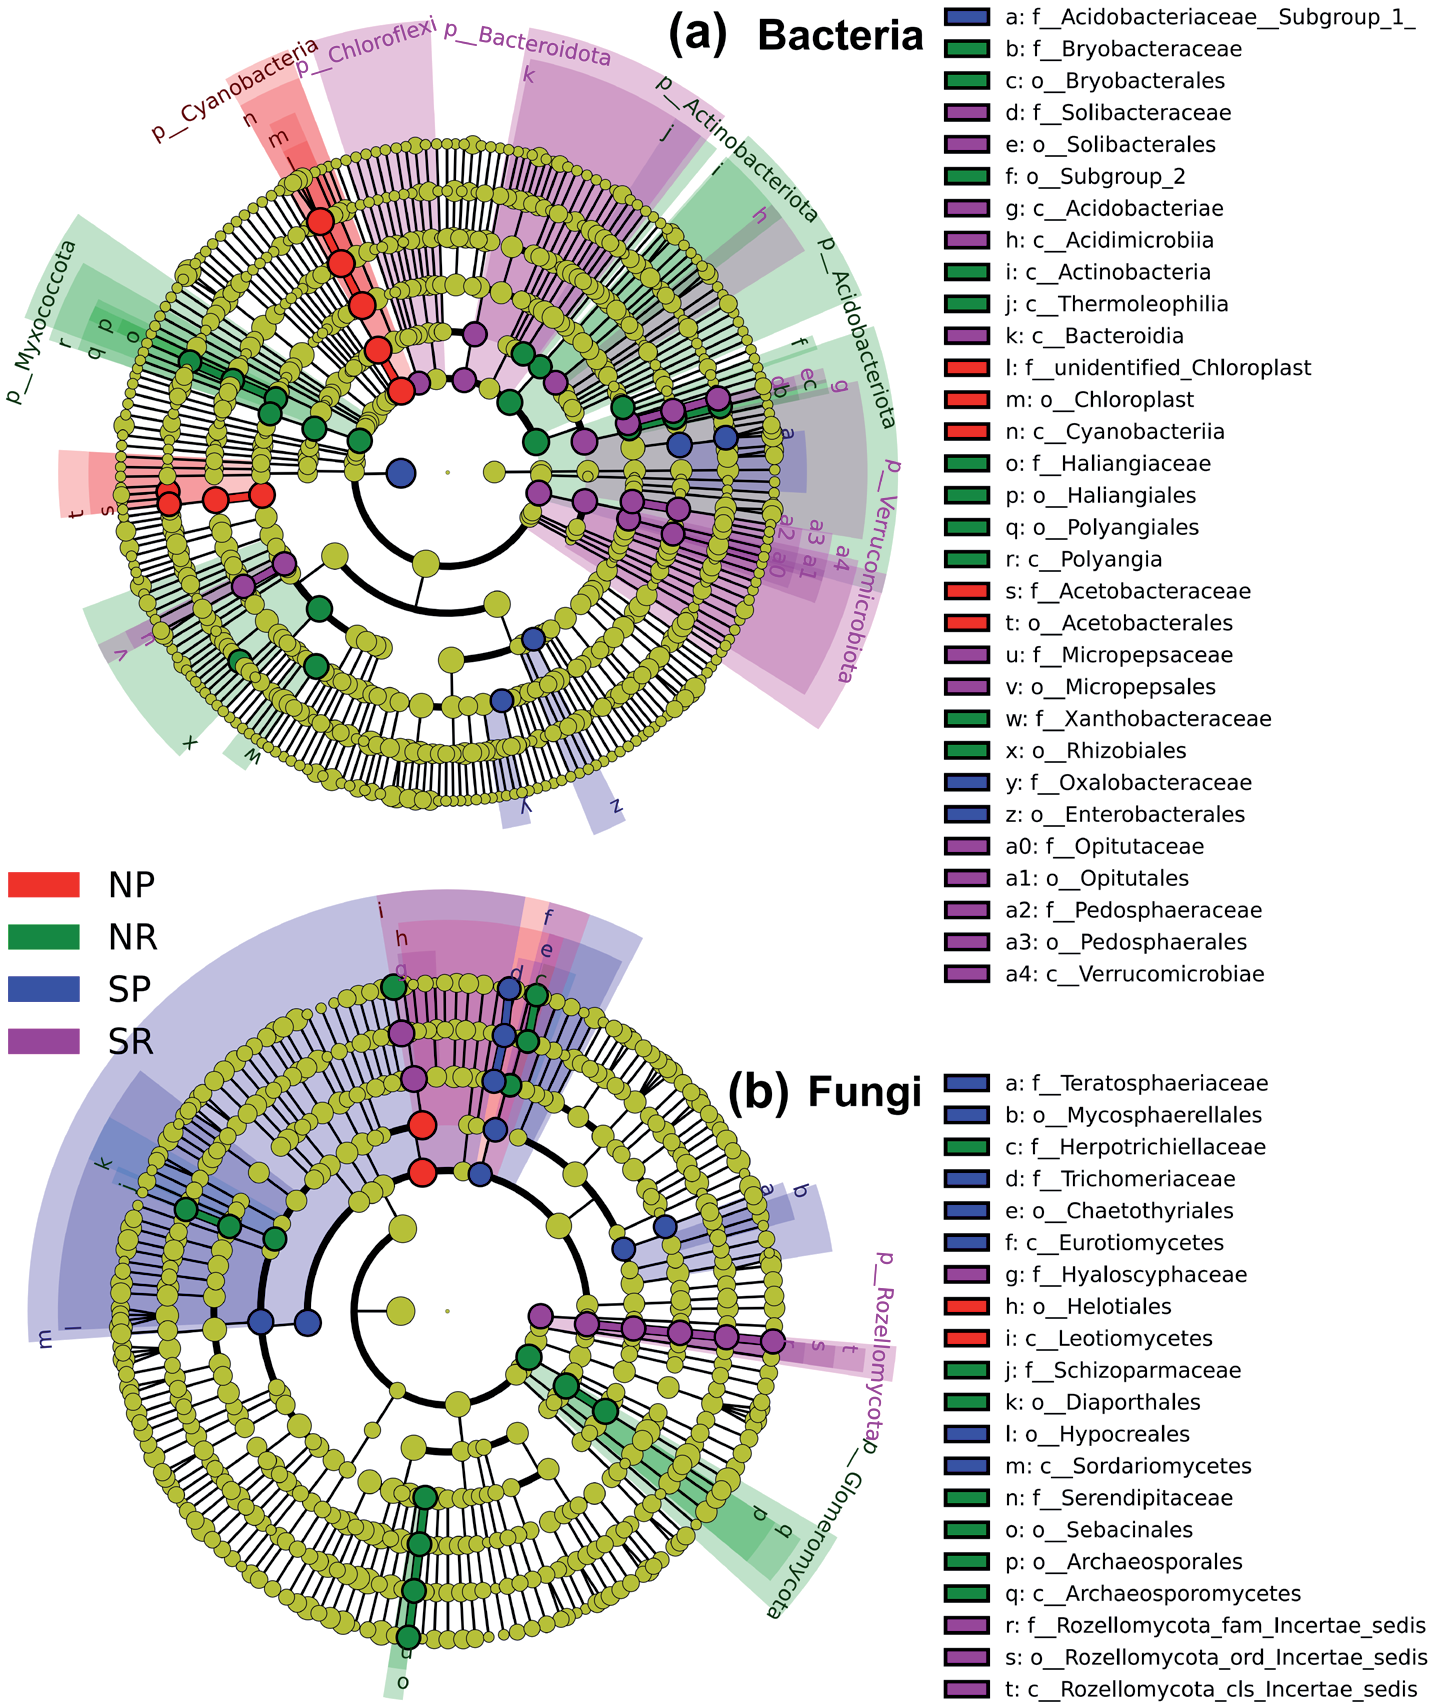
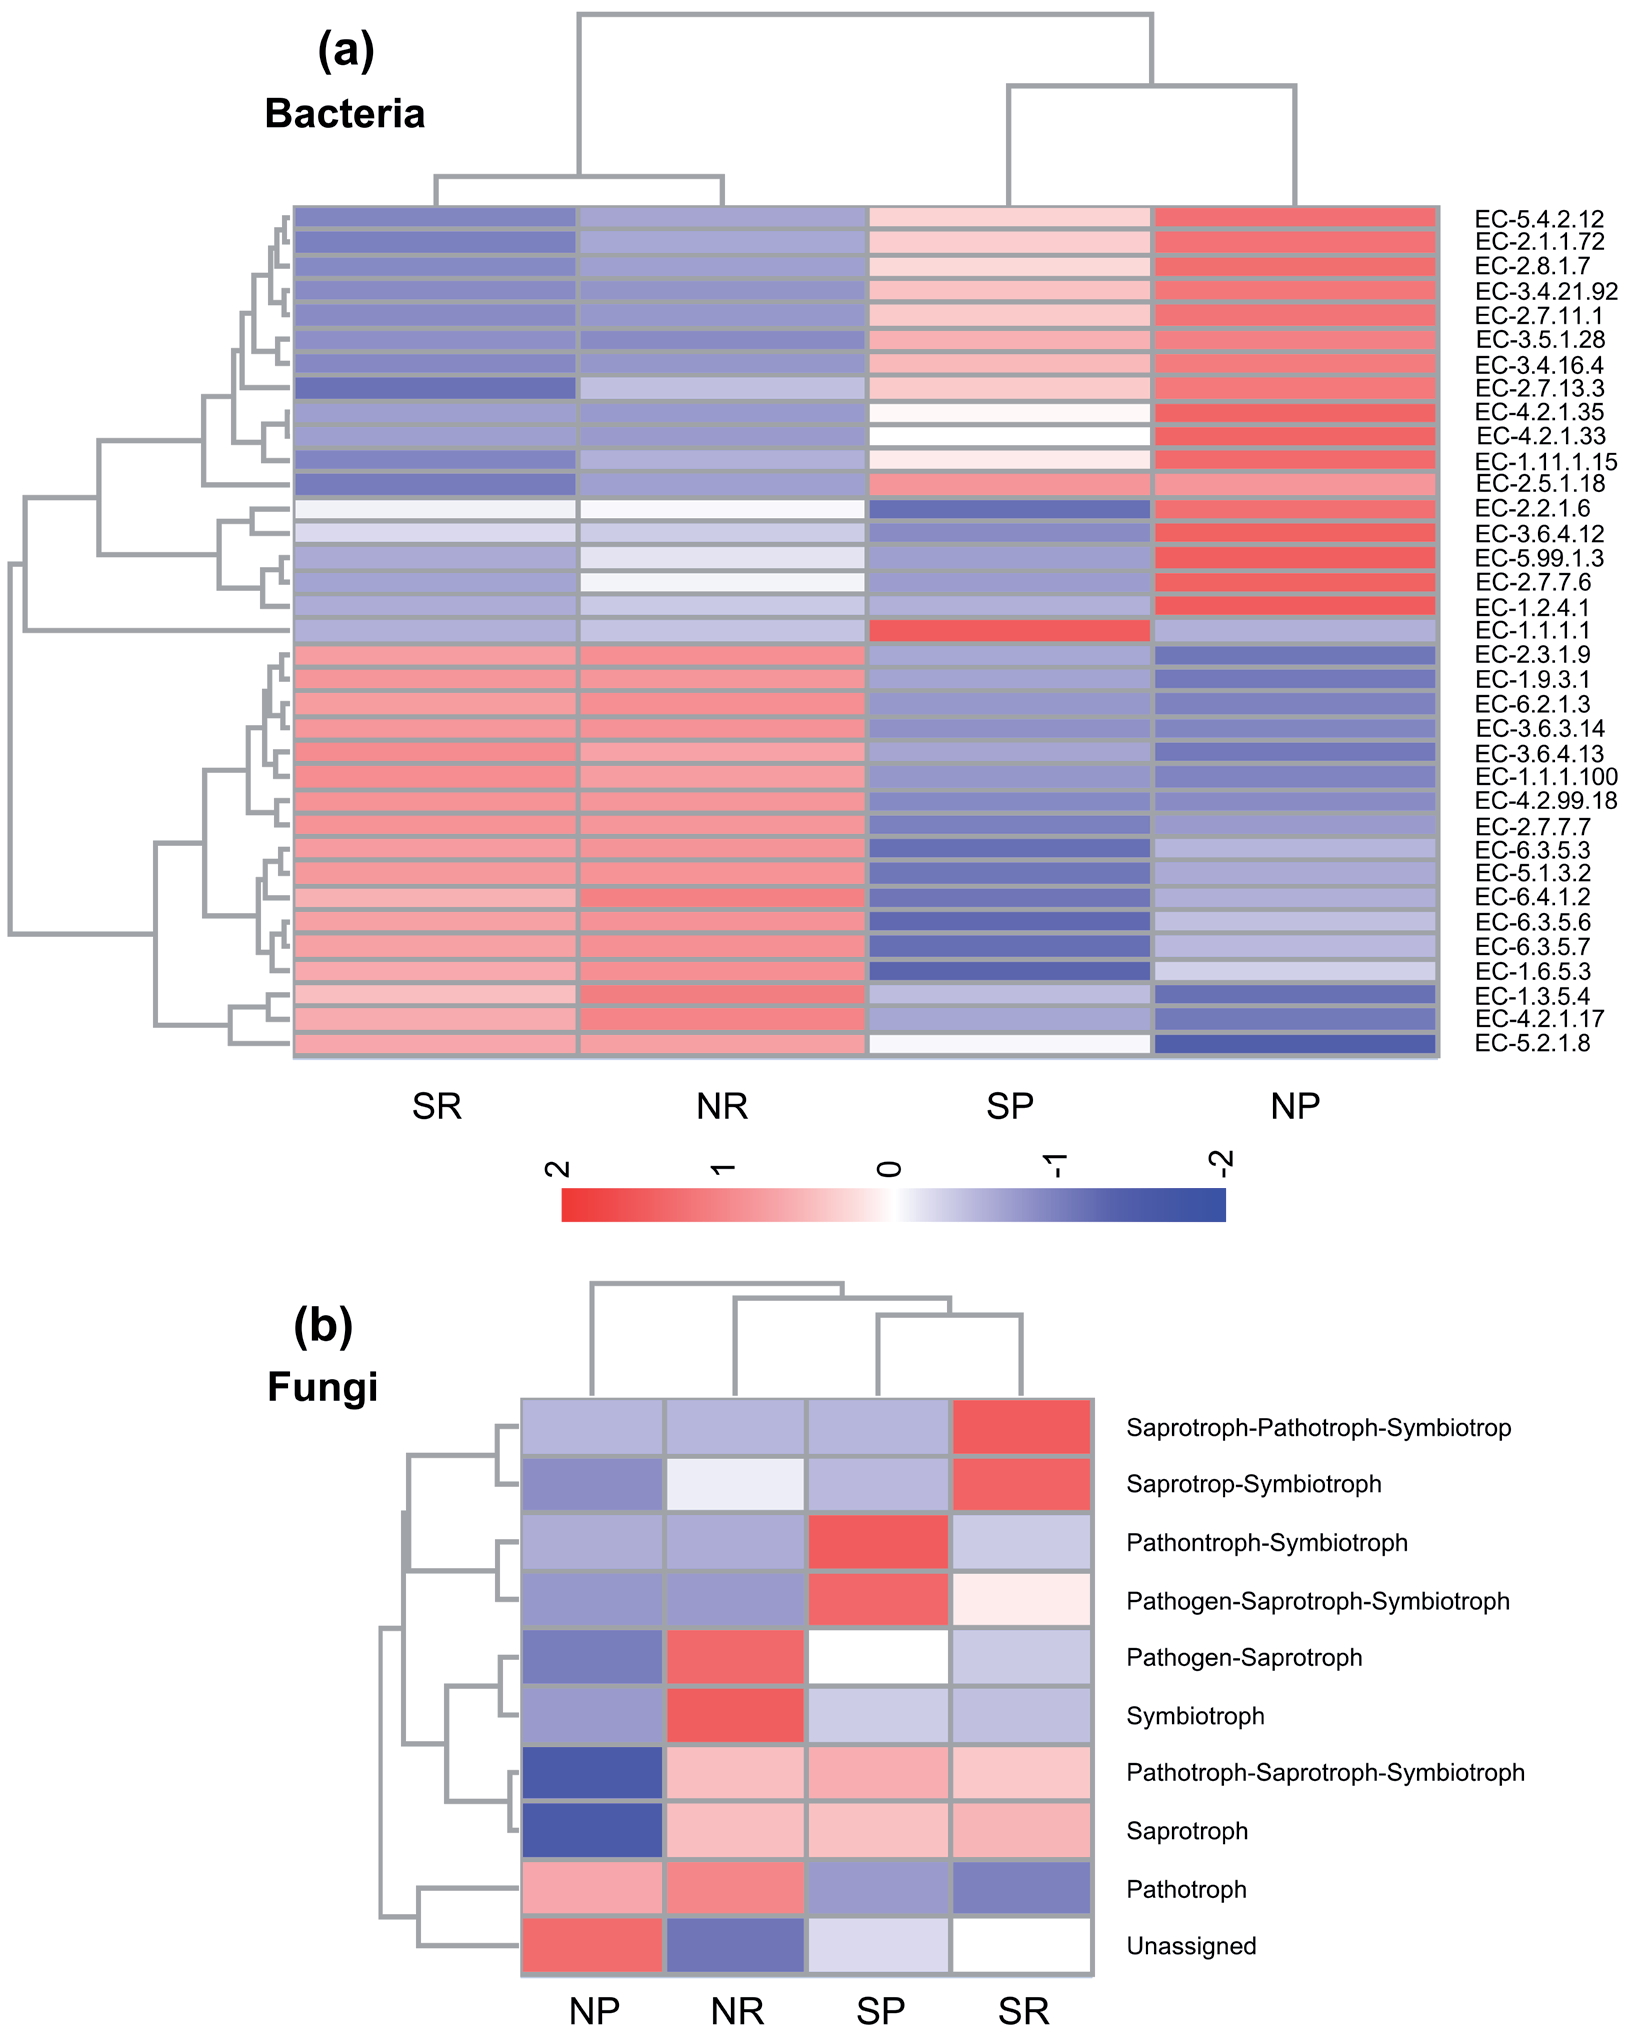
Restructuring the epiphytic microbial community by the shading not only occurred at the phyla level but also at the genus level (Fig. 5b, d). The heatmap diagram (Fig. 5) showed that the shading changed the relative abundance of the phyllosphere and rhizoplane bacterial and fungal genus. At the lineage level, LEfSe analysis of the bacterial community (Fig. 6a) found that five lineages were significantly enriched on moss phyllosphere under shading treatment, nine lineages on moss phyllosphere under non-shading treatment, sixteen lineages on moss rhizoplane under shading treatment, seventeen lineages on moss rhizoplane under non-shading treatment (LDA score ≥ 4, p< 0.05). LEfSe analysis of the fungal community (Fig. 6b) found that nine lineages were significantly enriched on moss phyllosphere under shading treatment, two lineages on moss phyllosphere under non-shading treatment, eight lineages on moss rhizoplane under shading treatment, fourteen lineages on moss rhizoplane under non-shading treatment (LDA score ≥ 4, p< 0.05). Collectively, partly in line with our first hypothesis (H1), the shading changed the phyllosphere and rhizoplane microbial community composition. The heatmap diagram (Fig. 7) showed that the shading changed the relative abundance of the phyllosphere and rhizoplane bacterial and fungal community functions. For bacterial communities, there was a clear distribution pattern of the abundance of genes encoding enzymes in the phyllosphere and rhizoplane (Fig. 7a); for fungal communities, the fungal mode distribution pattern differed among phyllosphere and rhizoplane, and shading and non-shading treatments (Fig. 7b). Besides, divergent network patterns were found (Fig. S2a-h), suggesting that shading changed the microbial network [50]. Collectively, the shading changed the phyllosphere and rhizoplane microbial community composition, function, and network, supporting our first hypothesis (H1). These alterations may have functional implications. Revealing their functional abilities is decisive for understanding their ecological significance [26]. Earlier research has shown the functions of moss-associated microbes. For instance, moss-associated microbes fix nitrogen, oxidize methane, and contribute to the decomposition of organic matter [51]. Moss-associated diazotrophs are assessed to supply more than 40% of nitrogen input to peatlands with a high accumulation of fixed nitrogen in vegetation biomass [52]. Moss‐associated methanotrophic bacteria can convert methane to CO2 [52]. In this study, the genera Burkholderia [46, 53], Trichoderma [47] (Fig. 5d), and Granulicella [46] (Fig. 5b) were typical inhabitants of moss. Most fungi in peatlands are saprophytes that participate in the decay of organic matter [48]. Over three hundred species of Ascomycota are found to parasitize mosses [30]. Mortierella and Cladosporium are opportunistic plant pathogens [30]. Saitozyma has a lignin-degrading capacity [54]. The alterations in the relative abundance of the bacterial and fungal genus would have significance for the elemental cycling, moss traits, and health.
Fig. 5.
Bar chart (a, c) and heatmap (b, d) showing the effect of shading on the phyllosphere and rhizoplane bacterial (a, b) and fungal (c, d) community composition at the phylum (a, c) and genus (b, d) levels, respectively. SP, moss phyllosphere under shading treatment; NP, moss phyllosphere under non-shading treatment; SR, moss rhizoplane under shading treatment; NR, moss rhizoplane under non-shading treatment.
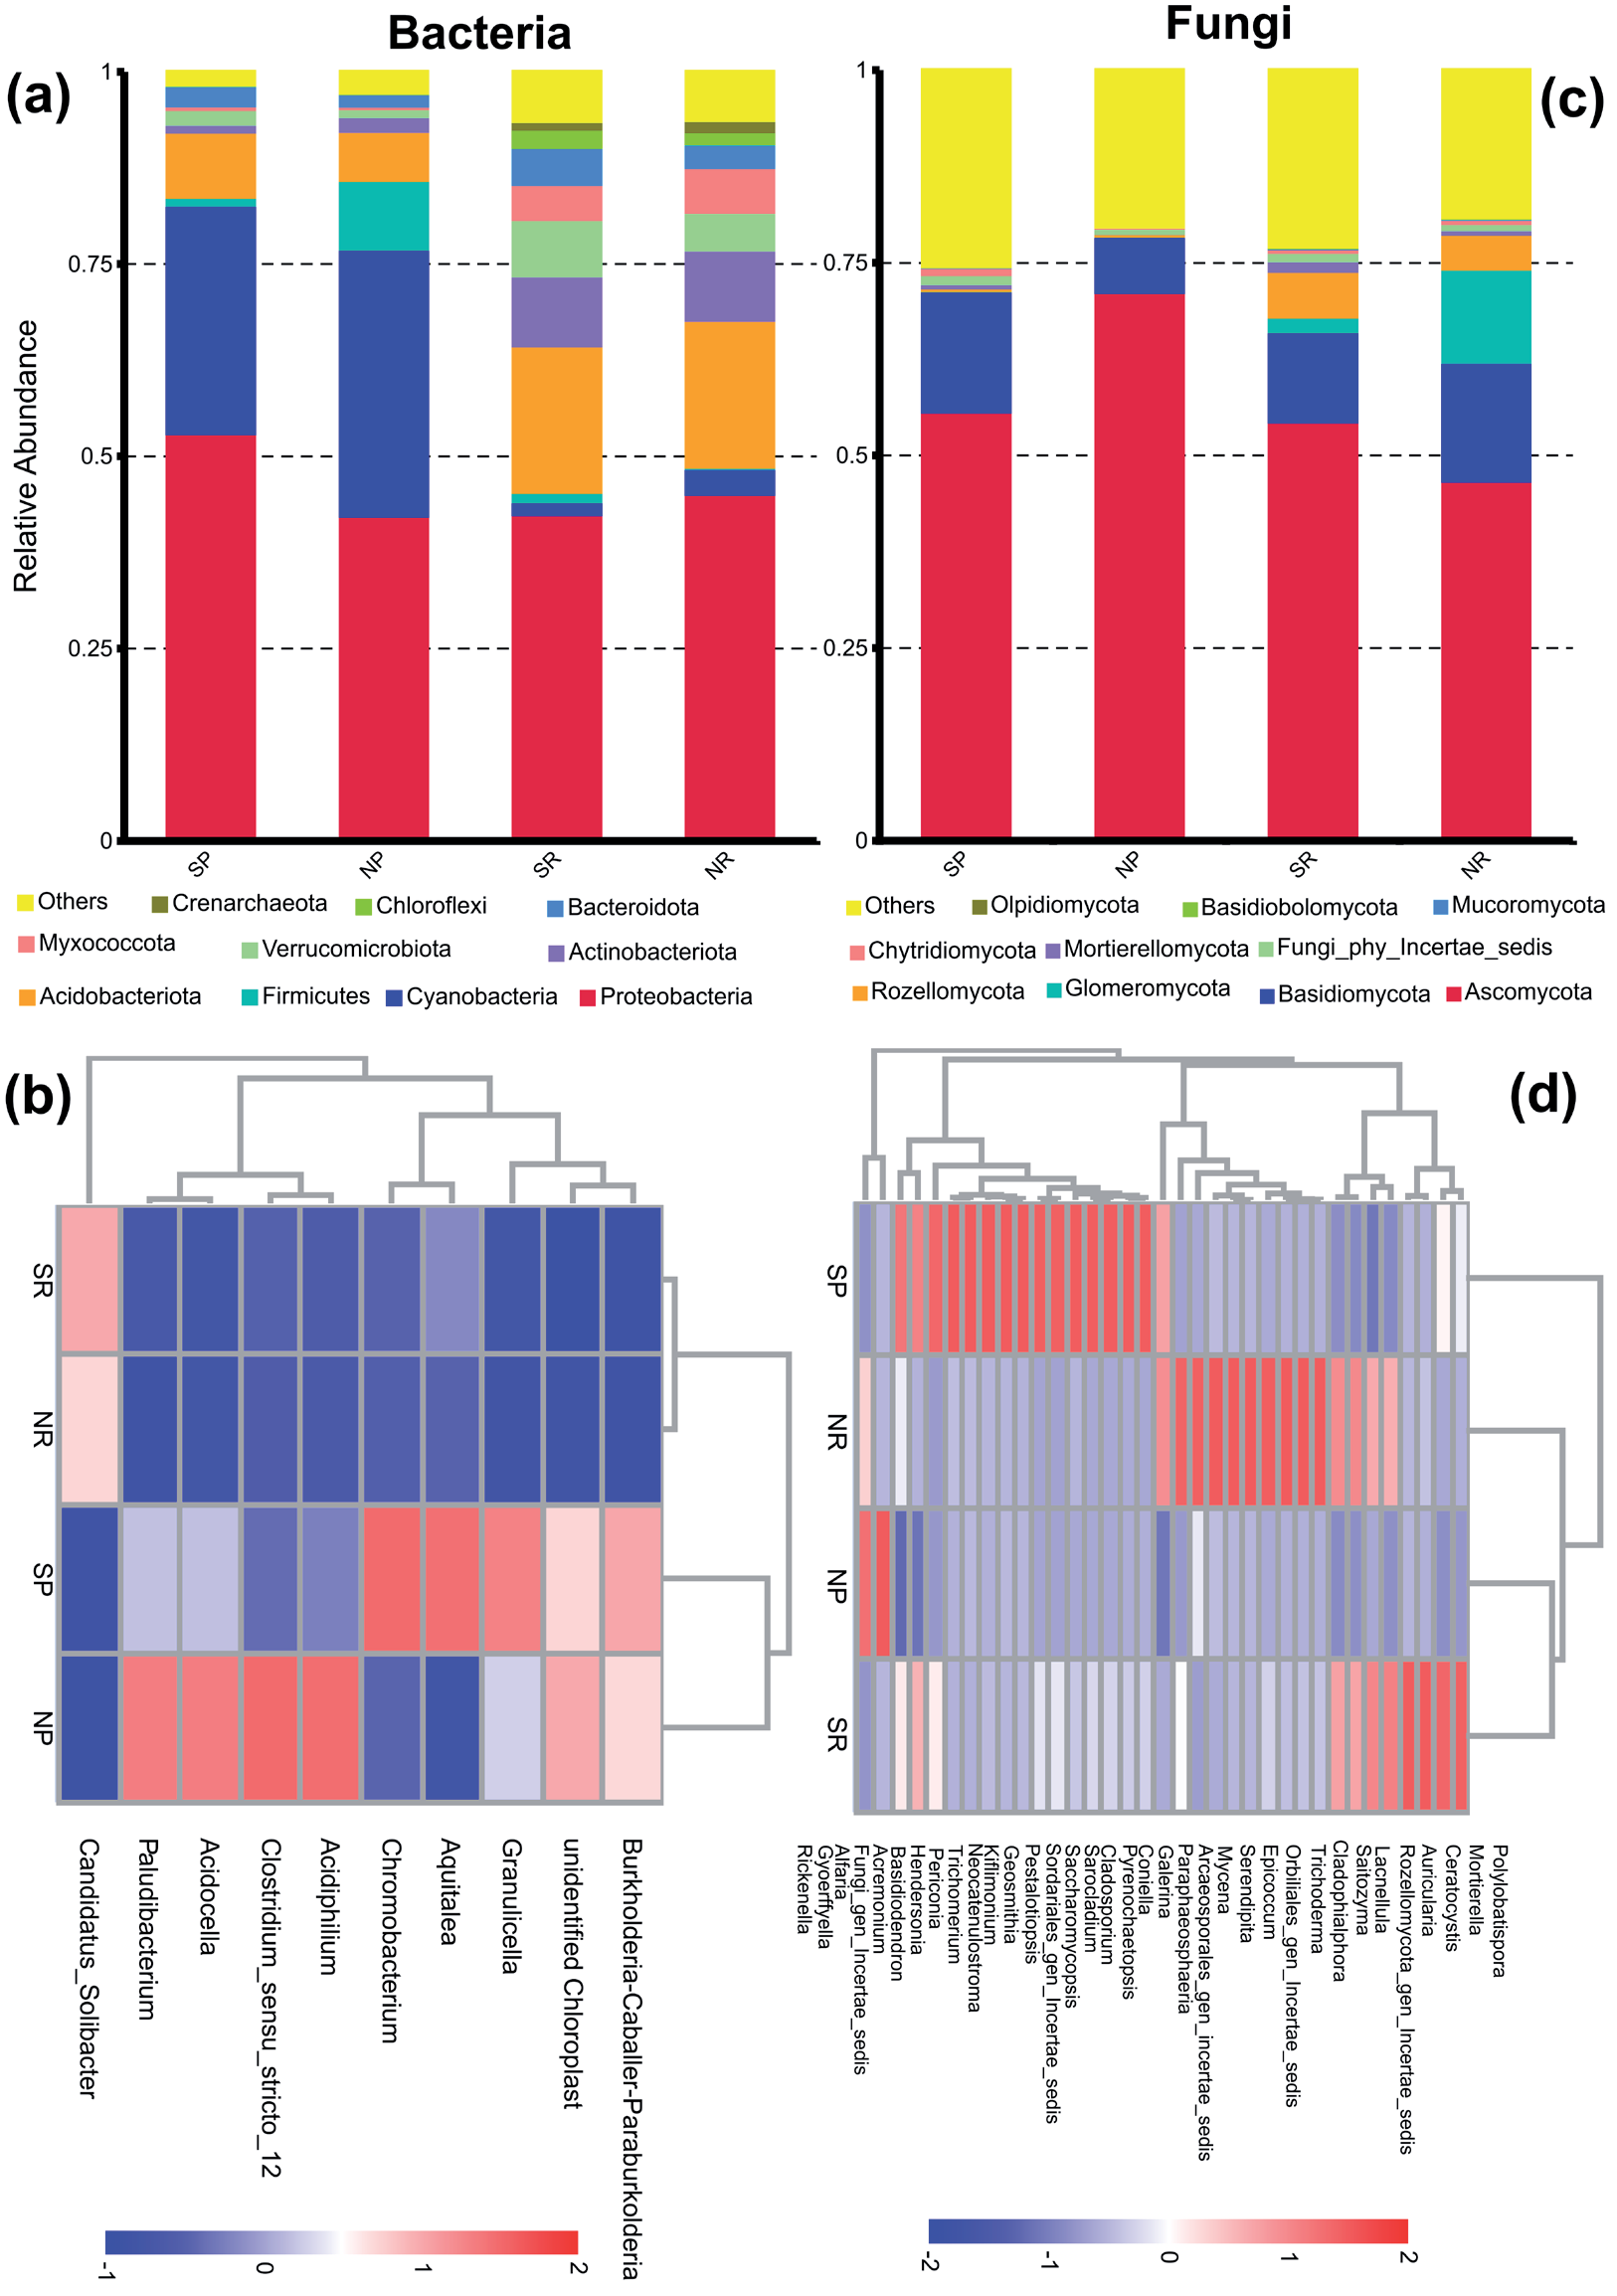
Fig. 6.
Cladogram showing the phylogenetic distribution of the phyllosphere and rhizoplane bacterial (a) and fungal (b) lineages and indicator with linear discriminant analysis scores (LDA) of ≥ 4 and p < 0.05 under shading and non-shading treatments. SP, moss phyllosphere under shading treatment; NP, moss phyllosphere under non-shading treatment; SR, moss rhizoplane under shading treatment; NR, moss rhizoplane under non-shading treatment.
Linking Phyllosphere and Rhizoplane Microbial Community to Moss Root Aluminum
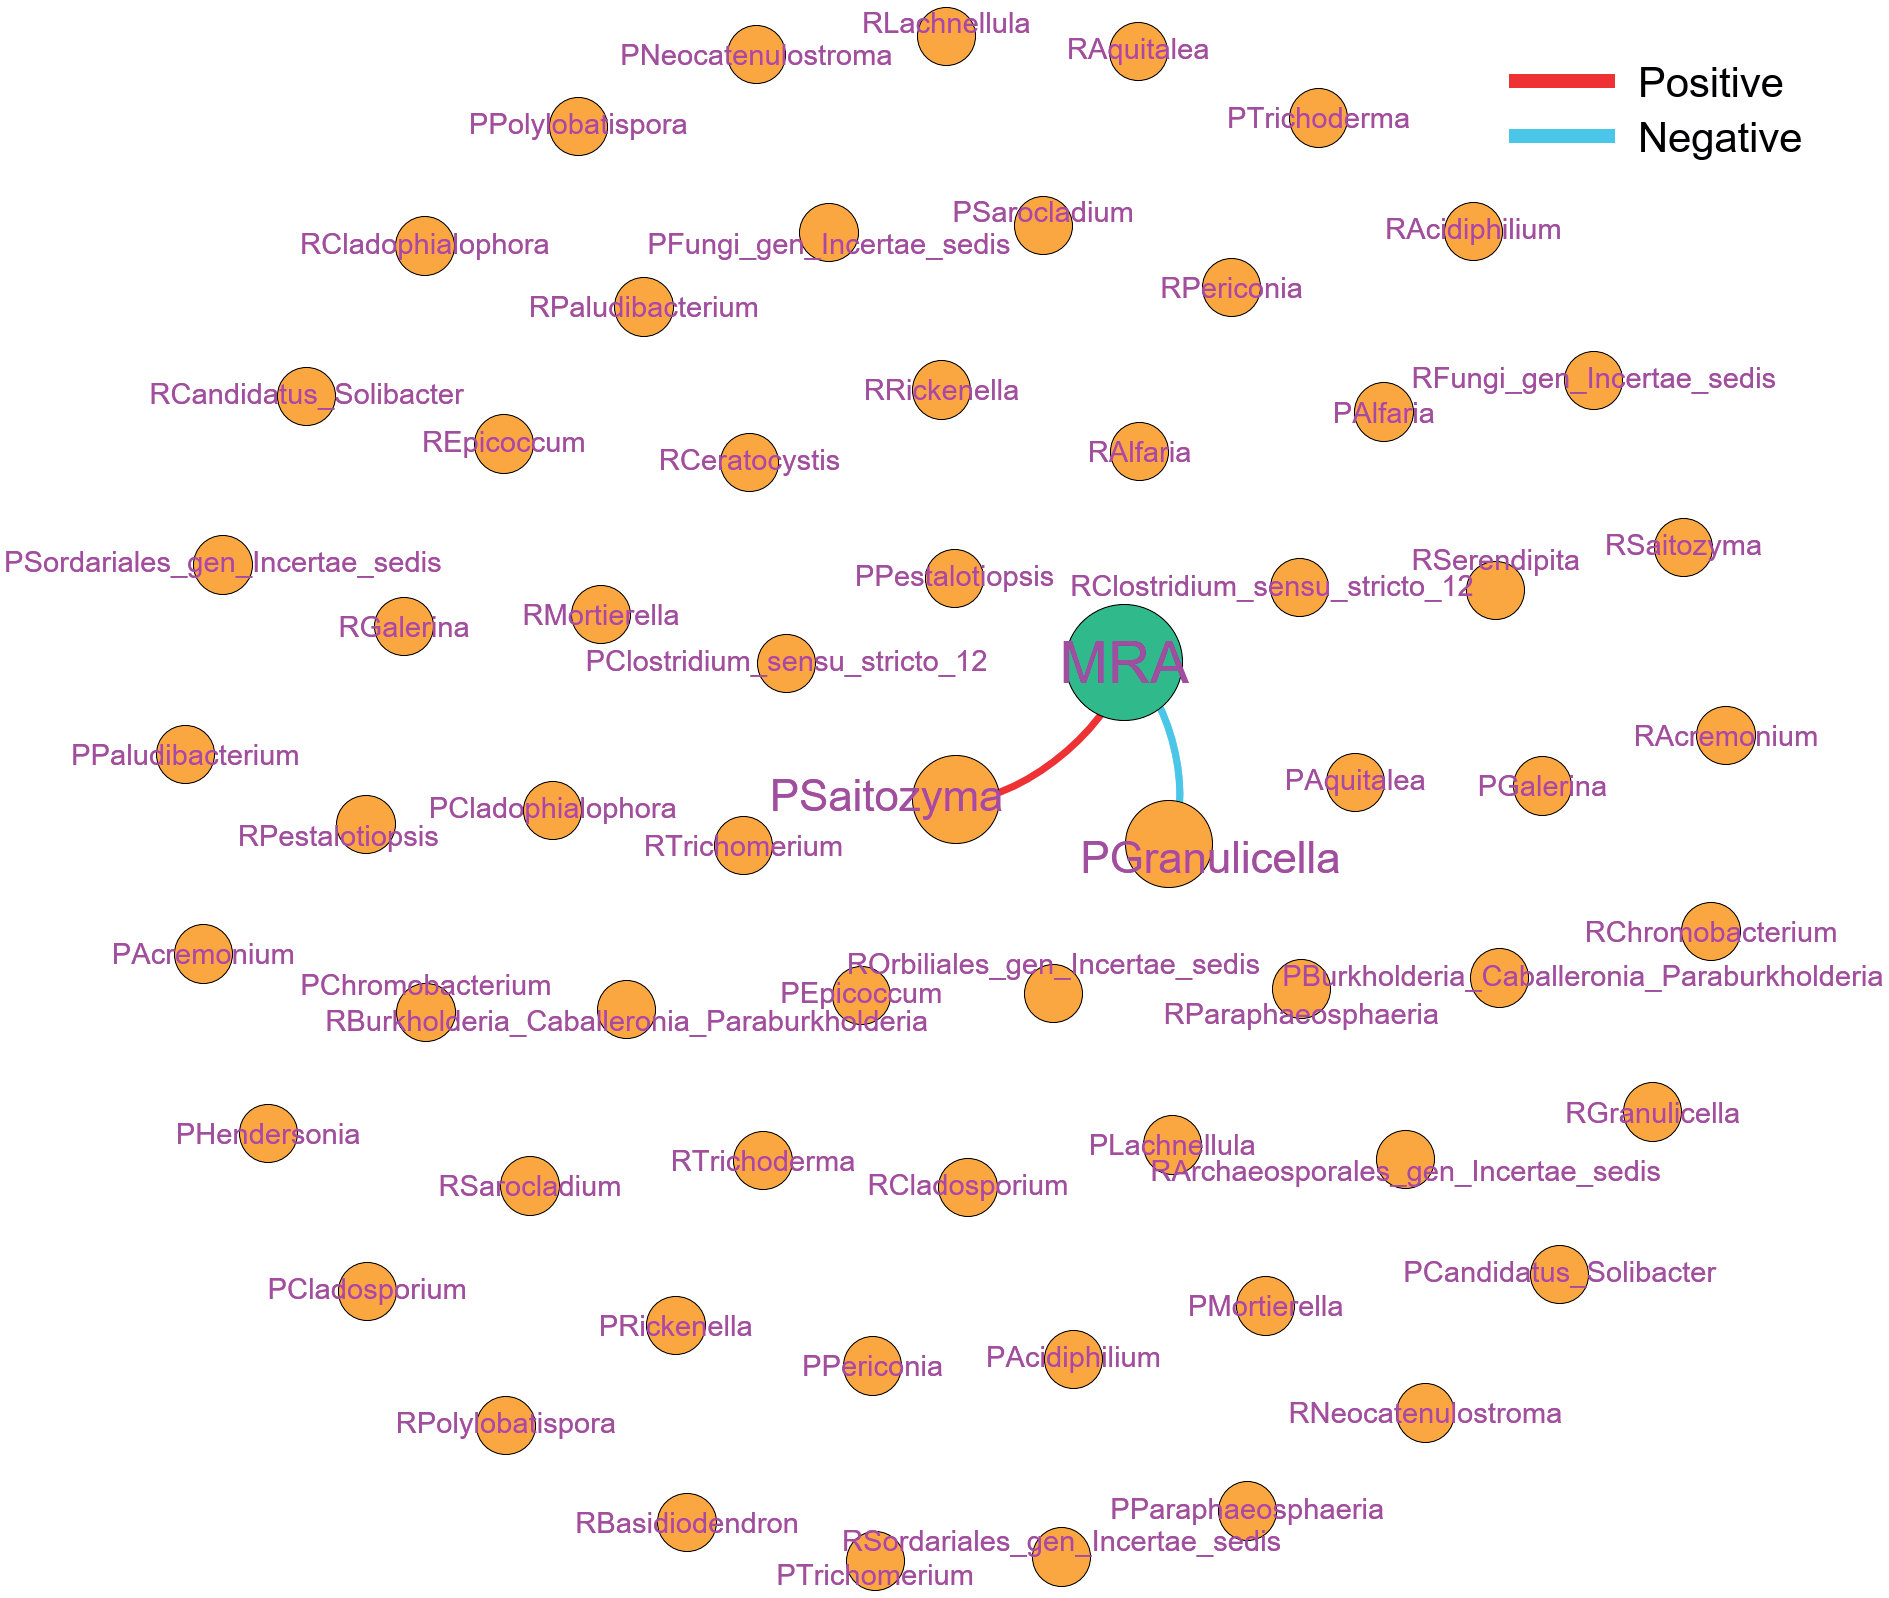
In the past, the growth and development of moss were influenced by soil water content, light and temperature, and nutrient availability [7]. Relationships between moss and fungus were long supposed to be uncommon [55]. However, in recent years, researchers have studied the feasibility of rapid artificial cultivation and restoration of moss and have gained some important findings [7]. For instance, moss manganese, iron, and molybdenum contents were positively related to moss-related soil biological nitrogen fixation and diazotrophic community [56]. In the present study, the bacterial and fungal community diversity (r = -0.3356 – 0.1557, p = 0.3431 – 0.9532, Table S2) and functions (r = -0.5505 – 0.5017, p = 0.09919 – 0.9918, Table S3) of the phyllosphere and rhizoplane were not significantly related to the moss root aluminum content. However, the higher relative abundance of the phyllosphere Granulicella genus (bacteria, Fig. 5b) and the lower relative abundance of the phyllosphere Saitozyma genus (fungi, Fig. 5d) under shading significantly facilitated the significant decline in the moss root aluminum content (Fig. 8, Table S4). A previous study showed that increasing temperature decreased the relative abundance of Granulicella [57]. The shading reduced temperature, which resulted in the higher relative abundance of the phyllosphere Granulicella genus under the shading. Granulicella is capable of utilizing various organic compounds [58] and degrading plant polymers [59] and toxins produced by the plant pathogenic fungus [60]. It is a potentially beneficial plant and a biocontrol microorganism [61]. Thus, the shading-induced higher relative abundance of the phyllosphere Granulicella genus was beneficial for moss. Furthermore, Saitozyma, a typical soil-borne yeast, was reported to suppress acetic acid fermentation [62, 63], and its occurrence was strongly associated with a high Al3+ [64]. The shading-induced lower relative abundance of the phyllosphere Saitozyma genus (fungi, Fig. 5d) was beneficial for moss. Ultimately, both decreased the moss root aluminum content growing in the acid soils. This finding has not been reported previously but rejects our second hypothesis (H2). The phyllosphere genus showed a tighter relationship with the moss trait than the rhizoplane genus did. This study emphasized the importance of the genus Granulicella and Saitozyma in shaping moss traits and updated the current knowledge regarding the positive interactions between moss and microbiome. However, the cause-and-effect mechanisms behind it remain understudied.
Fig. 7.
Heatmap diagram showing the effect of shading on the phyllosphere and rhizoplane microbial community function. SP, moss phyllosphere under shading treatment; NP, moss phyllosphere under non-shading treatment; SR, moss rhizoplane under shading treatment; NR, moss rhizoplane under non-shading treatment.
Conclusion
One year-shading sightly changed the soil physicochemical properties and most of the moss traits, whereas it significantly reduced the moss root aluminum content. The shading restructured the phyllosphere and rhizoplane microbial community composition, function, and network. The relative abundance of the Granulicella genus and Saitozyma genus of the moss phyllosphere were positively and negatively related to the moss root aluminum content. These findings will be useful for future improvements in moss production in southwest China.

