

Introduction
Sunflower seeds have multiple uses and can contribute as food, enhance aesthetic value, serve as biodiesel as a fuel source, and become a livestock feed source. Its oil is used as a raw material for the manufacturing of bioplastics, paints, varnishes, cosmetics, lubricants, soaps, and detergents [1]. Vegetative plant residues had a high concentration of potassium and phosphate that may be a substitute for organic fertilizer and improve the organic matter in the soil. The crop is grown in various world regions, including temperate, subtropical, and tropical climates, and is well adapted to a wide range of agro-environments. It is the 4th oil seed crop after palm oil, soybean, rapeseed, and mustard, with an average annual world production of about 52 MnT [2]. It accounted for 10% of the world’s production. However, production is concentrated in a few countries, such as Argentina, Ukraine, and Russia. These countries produce more than 60% of the total world production. The majority of the production comes from the European continent, i.e., Eastern Europe, Ukraine, and Russia, which produce 71% of the world’s production from 67% of the acreage under sunflower production.
Sunflower had a production of 58185.63 metric tons; an average per hectare yield was 1.97 tons, and globally, it was cultivated on an area of 29.532 million hectares. Russia (16.5 million metric tons) was the largest producer during the 2022 crop year, along with Ukraine (10 million metric tons), the European Union (9.48 million metric tons), Argentina (4.6 million metric tons), and Turkey (1.9 million metric tons) [3]. One of the production limitations is the absence of cultivars that are adapted to local conditions such as temperature and photoperiod. There is a continuous need for hybrids that may produce the maximum achene yield utilization in the local environmental and soil conditions. Sunflower hybrids offer many advantages for cultivation over open-pollinated cultivars, such as uniform maturity and easing harvesting. However, these hybrids are not adapted to local conditions marked with a specific range of agro-climatic conditions. The necessity for hybrids with distinct maturity groups has emerged with the expansion of agriculture into regions characterized by varying day lengths and temperature fluctuations.
The topic of the development of early maturing crop varieties is not new; however, it should be revisited under the scenario of global climate change. The benefits of early maturing crop varieties are enormous, and generally, early maturing crop varieties tend to escape from adverse conditions such as terminal biotic or abiotic stress conditions [4-6]. The maximum yield potential of a variety or hybrid may be obtained if it is phonologically adapted to a particular environmental condition [7]. Maturity time is known to be dependent on several factors, such as genotype, temperature, and photoperiod [8]. Photoperiod×temperature effect was significant from the seedling emergence to the initiation of floral buds. Photoperiod×accessions and temperature×accessions were also significant from days to seedling emergence and bud initiation and number of leaves. There was a delayed onset of reproductive phase initiation at 12 hours of light as compared to 14 hours of light, and this was due to poor photon flux density [9].
It was observed that high-yielding hybrids may exist in both early and late-maturing hybrids, and yield was determined by the total length period, from emergence to the floral anthesis, while oil contents were determined by the total reproductive period, and oil yield is determined by the total vegetative and reproductive period [10]. The longer vegetative phase allows greater production of photosynthates from the leaves due to a higher number of leaves and their leaf area index, while they may also have greater mobilization of stem reserves.
Studies in crop species such as soybean have shown that photoperiod along with thermal degree days may determine the days for floral initiation [11]. To lessen the influence on the environment, genotypes that are insensitive to temperature and daytime may be created. The sunflower flowering period was related to moderate additive variance and heredity [12]. For instance, several quantitative trait loci were known to affect the timing of flowering and, thus, maturity time in sunflowers, and these QTLs were also affected by environmental conditions such as photo-thermal conditions [13]. A total of 11 QTLs were identified on 10 linkage groups associated with the flowering time [14]. The hitchhiking genetic effects were found in the linkage groups 8 and 10. In another study, 6 QTLs in linkage groups A, B, F, I, J, and L were detected through a genetic linkage map of 205 RFLP loci for growing degree days to flowering [15]. A high degree of dominance variance was associated with days to floral initiation and days to 75% flowering, showing that hybrids differing with various maturity times may be developed by exploiting nonadditive variance, and selection may not be effective in segregating populations through phenotypic selection [16].
Studies have been carried out to identify breeding lines with good general combining ability, and accessions with negative combining ability effects have been preferred due to the carrying out of negative alleles related to days of flowering or days to initiation. It was hypothesized that accessions with negative alleles or negative combiners for days to flowering may reduce the time of flowering when utilized in breeding for early maturing hybrids. Inbred lines such as 20A (-1.27) and 23A (-0.76) were negative combiners for days to flowering but positive combiners for days to floral initiation and negative combiners for yield-contributing traits such as oil contents and achene yield per plant. These lines (20A, 23A) were positive combiners for protein contents [17]. Breeding lines COSF 10A (-1.40), COSF12A (-2.65), and COSF12A (-2.15) were negative combiners for traits such as days to flowering and days to maturity but had positive combining ability for oil contents and oil yield [18-20]. This study is designed to check the performance of different sunflower genotypes and the development of hybrids for different climatic zones.
Experimental Methods
Screening of the Parental Material
Sunflower elite accessions were evaluated for the days to 50% flowering, and 4 cytoplasmic male sterile lines, i.e., C-208, C-112, C-116, and C-124, regarded as “females” differing for the days to flowering, were mated with four testers, i.e., RH-344 (66 days), RH-347 (67 days), RH-446 (69 days), and RSIN-82 (66 days), regarded as “fertility restorer male lines”. These female and male lines were crossed with the line × tester (this analysis accurately predicts parents' general combining ability (GCA) and helps choose crosses with high SCA) fashion as narrated [21] to yield 16 single cross hybrids or half-sib progenies. To facilitate crossing, 2 rows of female lines were grown with 1 row of male. However, female and male lines differed in the time required to reach flowering. Therefore, female lines were synchronized by male lines about 10 days earlier than females. The female lines were planted as per their requirement for days to reach flowering to yield maximum F1 seed. Pollination was done manually by rubbing tissue paper on the male floral head, and then this tissue paper having pollen was gently rubbed with the female capitula having protruded receptive stigma. Male and female parents were maintained through sib mating by pollinating the heads of two plants within the same breeding line. F0 seed obtained from the female floral head was manually harvested and dried under shade. The seeds were cleaned all week, and unfilled seeds were removed. The seed was stored at room temperature. The seed was treated with insecticide before sowing in the field.
Crop Husbandry and Growth Condition
Sunflower breeding material from all crosses was sown at the research field of the College of Agriculture, University of Sargodha (Latitude: 32.13367° or 32°8'1" north; Longitude: 72.68705° or 72° 41' 13" east) during the spring crop season on 14th February 2022. A single seed was manually dibbled at a distance of 23 cm on both sides of the raised bed at a distance of 60 cm. Each row was about 6 meters long. There were 3 rows of each hybrid combination in a single replication. The fertility of the soil was increased by adding 2 bags of NPK (Engro Zarkhez 8:23:18) per acre. Soil moisture contents were determined by the gravimetric method by inserting soil at varying depths. Optimum soil moisture contents were about 18% by mass. No insecticide or fungicide was sprayed during the entire crop growth cycle. Weeds were controlled manually, and pre-emergence dual gold S-metlachlor was sprayed after sowing the seed of various hybrids. The experiment was sown in a randomized complete block, and there were three experimental blocks within the field. The experimental trial was evaluated for the following traits:
Day to 50% Flowering
Plants were visually scored after the formation of well-developed floral buds. The date of flowering was noted when at least 50% of the plant had opened flowers. Days to 50% flowering was the difference between the emergence and anthesis of 50% of plants within each row.
Plant Height (cm)
It was determined with the measuring tape from the base to the tip of the peduncle. All plants were evaluated, and an average of the 5 plants within each row was given in each replication.
Leaf Area (cm)
It was determined using the leaf area meter (LI- 3000C Portable Leaf Area Meter by LI-COR).
Head Diameter (cm)
Head diameter was determined with the measuring tape in the middle of the head from the front side. All plants were evaluated, and an average of the 5 plants within each row was given in each replication.
Seed Yield (g m-1)
The seeds of the six plants within each row were manually threshed, and seed moisture contents were reduced to 12% by drying in the oven. Afterward, seed mass was determined on the digital balance, and the value was given in g m-1.
Dehulling (%)
100 g of the seed was dehulled, and kernel mass was determined on the digital balance. Dehulling % was determined as follows:
Kernel Oil (%)
Kernel oil contents were determined with the Soxhlet apparatus using hexane as a solvent [22].
100-Seed Mass
100 seeds were counted on the seed counter, and the mass of 100 seeds was determined on an analytical balance.
Fatty Acid Profile
It was determined over the gas chromatography machine. Oil (50 µL) was methylated using 4 ml KOH (CAS No: 1310-58-3) for 1 hour at room temperature. The methylated fatty acids were extracted with hexane (Catalog Number: 11392357). The analysis is done by using the fused capillary column, flame ionizing detector, and nitrogen gas carrier at 3.5 ml min-1. Injector and detector temperatures were set at 260°C, while column oven temperature was set at 222 °C. Methylated esterified fatty acid is injected manually, while fatty acids were identified through peak retention time when compared with the standard.
Statistical and Biometrical Analysis
Analysis of variance was carried out in “R” computer-based software using the library “doe-bioresearch” using the function “frbd2fact”. Analysis of variance was carried out in a randomized complete block design with two factors and three blocks. Genotypic and phenotypic correlations were also estimated through the library “variability”. Genetic analysis of days to flowering was carried out over two years. The analysis was done in “R” using the function “gpbStat”.
Results
Analysis of Variance
Analysis of variance showed significant variation among accessions for days to flowering. Elite sunflower accessions were evaluated for days to flowering, and germplasm was characterized as late flowering, which included accessions, i.e., RH-447, RHA-455, and RFSS- 88. These accessions reached floral anthesis in 68- 69 days (Fig. 1). Accessions B-124, RHA-344, B-259, RHA-345, and B-224 65-66 days. Accessions B-2721, RH-365, B-249, B-116, B-243, B-2721, and B-112 reached anthesis in 63-64 days. Accession, i.e., B-208 (62 days), B-65 (61 days), B-11-278, and B-249-2728 (58 days), took the lowest number of days to reach anthesis and thus are considered the earliest. Selected female accessions, i.e., C-112 (63 days), C-116 (64 days), C-124 (66 days), and C-208 (62 days), differing for days to flower, were mated with four male fertility restorer lines (RH-344 66 days), RH-347 (67 days), RH-446 (69 days), and RSIN-82 (66 days) to yield 16 cross combinations or half-sib progenies. Analysis of variance showed highly significant variation due to cross combinations, years, and cross combinations×years (Table 1).
Cross combinations showed insignificant variation during the years 2022 and 2020 (Table 2). However, females showed significant variation in both years, and males showed insignificant variation during both years. Interaction between females×males was insignificant during the year 2022 and significant during 2020 (Table 2). Heritability was low during the year 2022 but medium during the year 2020. Moreover, the contribution of epistatic and dominance was highly associated with genotypic variance for days to flowering (Table 2).
The range of the cross combination for days to flowering was 54-62. Cross combinations C-208×RH-344 and C-116×RH-344 were the earliest, while combinations C-112×RH-344 and C-112×RH-347 showed late flowering (Table 3). The ranking of the hybrids changed over the years, showing that days to flowering have a significant impact on the years. Factors such as photoperiod and thermal degree days significantly influence the days to flowering, and numerous quantitative trait loci have been mapped in sunflowers that affect the flowering time in sunflowers.
Fig. 1.
Variation among sunflower elite accessions for days to flowering. A least significant test (LSD) was applied. Different small letters (a, b, and c) above the column differ at p < 0.05.
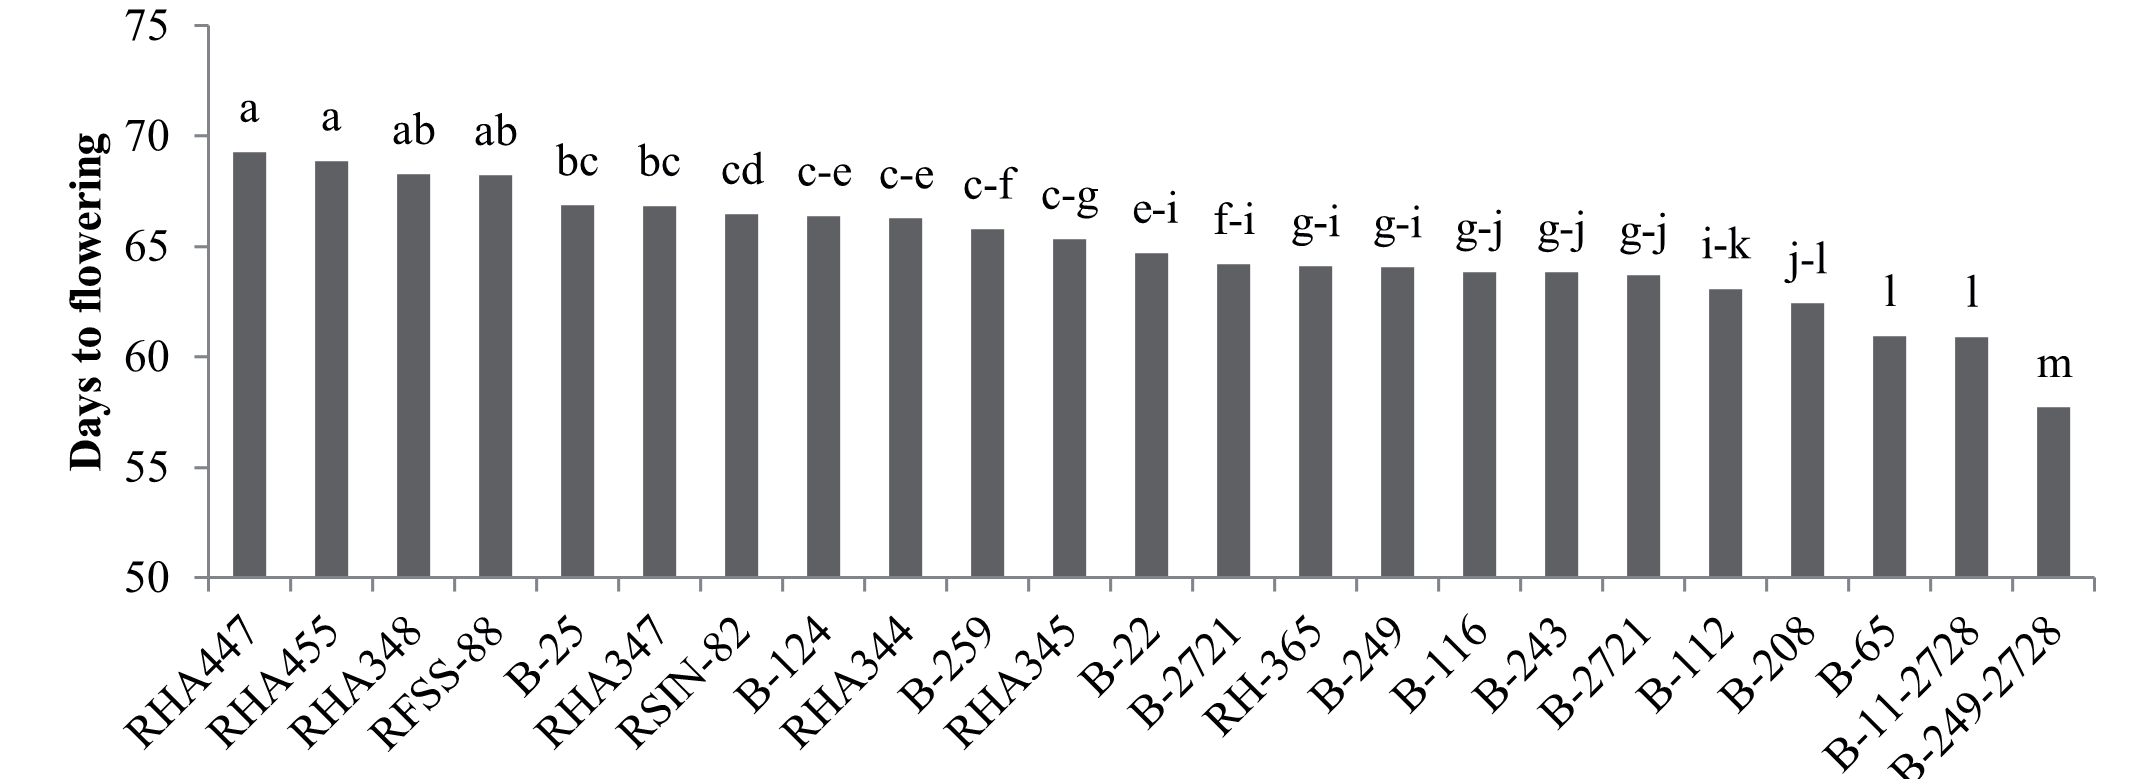
Table 1.
Analysis of variance and genetic components within years (2020-22).
Breeding lines such as C-208 and C-116 were useful parental lines for breeding early-maturing hybrids, as these breeding lines had significant negative general combining effects in both years (Table 4). Among male parents, RH-344 and RH-347 were negative general combiners and could be exploited to produce early maturing hybrids (Table 4). Breeding lines B-112 and RSIN.82 were good positive general combiners for the development of late-maturing hybrids.
Cross combination C-124 × RH-456 had the highest negative specific combining ability effect. Similarly, cross combinations C-112×RSIN.82, C-116×RH-347, C-116×RH-344, C116×RH-347, C112×RH-347, and C-208×RH-344 also had negative specific combining ability effects for days to flowering and thus may be considered for the development of early maturing hybrids.
Correlation
Genotypic correlation has been presented in Table 5. There was a positive relationship between days of flowering and head diameter. The relationship (P ≤ 0.05) between days of flowering and seed yield was also positive. The positive relationship of days to flowering between the head diameter and seed yield shows that hybrids with later flowering had higher yield potential under non-stress conditions. As far as phenotypic correlations go, days to flowering had an insignificant relationship with any of the parameters under study (Table 6). Higher leaf area was a positive contributor with yield parameters such as 100-seed mass and leaf area (Table 5, 6).
Table 2.
The mean value of various cross combinations during the years 20-22.
Mean Values
Head diameter (HD) ranged between 21–25 cm. The HD of all cross combinations was statistically similar, and there were no differences among the late and early maturing hybrids except C-116×RH-344, which had significantly lower HD than all other hybrids (Table 7). 100-seed mass ranged between 4–6 g. Early maturing had a 24% higher 100-seed mass than late maturing hybrids. Cross combination C-208×RSIN-82 had the highest 100-seed mass (Table 7). Leaf area ranged from 576–852 cm2. Early maturing hybrids had 8% higher leaf area than late maturing hybrids. The leaf area of their medium maturing cross combination (C-124 × RH- 344) was the highest. Achene yield ranged between 231– 316 g m-2. Late-maturing hybrids had a yield advantage of 17% over early-maturing hybrids. Cross combination C-112×RH.456 had the highest achene yield (g m-2) (Table 7). Days to 50% flowering ranged between 53– 61 days. Cross combinations of C-116×RH-344 had the lowest days to 50% flowering, while late-maturing hybrids C-112×RH-456 had the highest days to 50% flowering. Later-flowering hybrids had about 8% more days to flower. Hybrid physiological maturity ranged between 94–110 days. C-112×RH.456 took the highest number of days to reach maturity, while C-16×RH-344 had the lowest days to reach physiological maturity (Table 7).
Table 4.
Specific combining ability effects for days to flowering in the years 2020-22.
Table 5.
Genotypic correlations among various morphological traits related to seed yield.
Table 6.
Phenotypic correlations among various morphological traits related to seed yield.
Oil Contents and Morphological Traits
Kernel oil contents ranged between 42–51% for various cross combinations under study. The cross combinations C.208×RH.344, C208×RSIN.82, and C112×RSIN.82 had the highest kernel oil contents (Table 8). Early maturing hybrids had 5% more kernel oil content than the late maturing hybrids. Oleic acid contents ranged between 35–80%, and cross combinations C.112×RH-344, C116×RH-344, C112×RH-347, and C112×RH-456 were hybrids with high oleic acid contents. Combinations C-208×RH-344 and C124×RH-344 had medium oleic acid contents. C-208×RSIN.82 had low oleic acid content. Dehulled kernel % ranged between 43–61%. Early maturing hybrids had 43% higher dehulled kernel % than late maturing hybrids. C116×RH-344, C208×RSIN.82, and C208×RH.344 had the highest dehulled kernel % (Table 8). Kernel yield ranged between 121–157 g m-2. Early hybrids had a kernel yield advantage of 10% over later-maturing hybrids. Cross combinations C.116×RH-344, C.208×RSIN82, and C-112×RSIN.82 had the highest kernel yield, while C112×RH347 had the lowest kernel yield (g m-2). Oil yield rating between 57–80%. Early maturing hybrids had an oil yield advantage of 7% over late maturing hybrids. C-112×RSIN.82 and C-208×RH.344 had the highest oil yield and may be considered for general cultivation (Table 8).
Discussion
Elite breeding lines studied in our trial were evaluated for days to flowering, and germplasm was characterized as late flowering. Days to flowering have been affected by various environmental conditions, such as temperature and photoperiod. Studies in sunflowers showed variation in flowering days as per the location of the study. There was wide variability among the sunflower hybrids for their time of maturity, which ranged between 86 days and 98 days in Iran [23]. However, the mean days to flower in 38 sunflower hybrids were about 113 days under temperate conditions in Islamabad, Pakistan [24]. The coefficient of genotypic and phenotypic variation was low for days to flowering and days to maturity, which was about 95 days [25]. Days to flowering in 32 germplasm accessions ranged between 57–70 days at the Oilseed Research Station in India [26]. In Romania, a study was conducted to determine the floral initiation of 17 sunflower hybrids at five locations during the years 2018-19, and it was shown that the average of the 17 hybrids was about 59 days during the year 2018 and 66 days during the year 2019 [27]. Floral initiation ranges were 56–62 and 61– 68 days during the years 2018-19 [27]. Days to 50% flowering of 28 sunflower hybrids ranged between 57– 77 days at Vijayapura, India, and negative heterosis over the standard check ranged between -9.72–-25 % [28]. Days to 50% flowering ranged between 84–103 days, determined at Holeste, Edisababa, Ethiopia. The mean days to 50% flowering of 25 sunflower accessions were 95 days [29]. In this study, cross combinations also took 53-61 days for flowering, consistent with the previous findings. However, the genotypic coefficient of variation within days of flowering was low across many studies, which indicated accessions were similar for this important trait. Therefore, breeding for sunflowers with different maturity groups may be required.
Table 7.
Mean values over two years for traits related to yield and other morphological traits.
Table 8.
Mean values over two years for traits related to oil yield and other morphological traits.
Knowledge regarding the genetic parameters and type of variation associated with traits of interest may be required for the exploitation of genetic variation through various breeding schemes. The total genetic variance contribution to the phenotypic variance of earliness was about 54%, followed by the environmental variance contribution (estimated from three locations in Baluchistan, Pakistan), which was 22.47% [30]. A high degree of dominance variance was associated with days to floral initiation and days to 75% flowering, showing that hybrids differing with various maturity times may be developed by exploiting nonadditive variance, and selection may not be effective in segregating populations through phenotypic selection. A study showed that days to floral initiation and days to 100% flowering had additive types of genetic variance, and thus, it may be selectable by phenotypic selection [31].
Our study, which was conducted over two years, indicated that cross-combinations showed insignificant variation between 2022 and 2020 (Table 2). However, females showed significant variation in both years, and males showed insignificant variation. Interaction between females×males was insignificant during the year 2022 and significant during 2020 (Table 2). Heritability was low during the year 2022, but medium during the year 2020. Moreover, the contribution of epistatic and dominance was highly associated with genotypic variance for days to flowering (Table 2). Therefore, pedigree selection for the establishment of pure lines may not be possible due to a lack of additive variance and a preponderance of dominance or epistasis associated with days to flowering. Moreover, the genotypic coefficient of variation was also present in both years, as indicated in many studies conducted earlier. Therefore, recurrent selection may be practiced to develop breeding lines specifically with different maturity groups. Selection may be practiced in developing populations with varying maturity and to break intra or inter-allelic interactions. However, overdominance may also be exploited in the F1 generation by crossing suitable breeding lines to develop early or late-maturing hybrids. Breeding lines such as C-208 and C-116 were useful parental lines for breeding early-maturing hybrids, as these breeding lines had significant negative general combining effects in both years (Table 4). Among male parents, RH-344 and RH-347 were negative general combiners and could be exploited to produce early maturing hybrids (Table 4). Breeding lines B-112 and RSIN.82 were good positive general combiners for the development of late-maturing hybrids. A comparison between early and late-maturing hybrids under study showed that late-maturing hybrids had superior achene yield due to a prolonged growth period, which may have increased the total degree required for maturity. However, early maturing hybrids had higher oil contents, greater kernel seed yields, and kernel-to-achene % and thus had higher oil yields, which may be due to the voidness of terminal heat stress, which may have increased the oil yield potential of early maturing hybrids. However, late-maturing hybrids also had a higher achene yield. The development of sunflower hybrids with various maturity groups is essential for adapting to the caring lengths and conditions of diverse seasons. Sunflowers require seasonal adaptation to specific temperatures and daylight hours to produce seeds and optimal growth. Different maturity periods of hybrids allow planting all over the year, getting the most out of yield potential through seasons, and in risk management, the early-maturing hybrids can be harvested before frost or heavy rains, reducing the risk of loss. Hybrids of late maturation offer higher yields in longer seasons.
Sunflower cultivation success heavily relies on choosing the right hybrid for the specific season and region. Sunflower hybrids with distinct maturity groups optimize their adaptability to various seasons. In seasonality, different seasons present unique challenges, like temperature fluctuations, daylight hours, and precipitation patterns. Early hybrids mature quickly and are ideal for short growing seasons or late planting; however, late hybrids offer higher yields but require longer daylight and warmer temperatures. While in regional variations, climate conditions vary considerably across regions, necessitating hybrids suited to specific environments. Drought-tolerant hybrids might be crucial in arid zones, while cold-resistant ones are vital in regions with early frosts. Oil constant and quality variation in maturity groups can influence oil content and quality. Early hybrids might sacrifice some oil content for quicker maturation; however, late hybrids can offer higher oil yields but lower quality due to potential over-ripening. Sunflower production thrives across a range of climates and seasons, but optimizing harvest depends on selecting the cultivars with appropriate maturity groups. During the seasonality, each region experiences unique temperatures and sunlight patterns throughout the year. However, short growing seasons require early-maturity hybrids, while longer seasons allow for later-maturing varieties with potentially higher yields. The sunflower maturity groups cultivars are classified into maturity groups based on the number of days from planting to seed maturity. Early hybrids mature in 75 to 90 days, while late hybrids may take 120 to 130 days.
Conclusions
The success of sunflower production mostly depends on selecting the appropriate hybrid for the local climate and time of year. Sunflower hybrids that belong to different maturation groups are best suited to different seasons. Seasonality refers to how distinct challenges, such as variations in temperature, daylight hours, and precipitation patterns, are presented by the several seasons. Early maturing hybrids like C-208 × RH-344 exhibit superior early maturity and might potentially be commercialized to mitigate the effects of climate change. Future studies must focus on field evaluation of these cross combinations under different climatic conditions and the optimization of agronomic practices such as planting density, irrigation regimes, and nutrient management specifically tailored for early-maturing hybrids.
Authors Contribution
Muhammad Arslan and Saeed Rauf designed the study. Muhammad Arslan, Rao Muhammad Samran Gul, Waqas Khalid, Maham Nazish, Muhammad Anwar, Taiyyibah Basharat, Adeel Anwar, Sajid Fiaz, and Muhammad Uzair perform the experiments and data analysis. Muhammad Arslan, Muhammad Uzair, and Sajid Fiaz helped with data analysis, software standardization, and the writing of the original draft. Abdel-Halim Ghazy, Abdullah A. Al-Doss, Kotb A. Attia, Muhammad Uzair, and Saeed Rauf provided technical expertise to improve the article and helped fund acquisition. Saeed Rauf supervised the whole study. All authors reviewed and edited the manuscript.

