

Introduction
The vascular cambium is the most extensive meristem in the tree and is continuous and unbroken from the top of the tree to the roots. It is defined as the actively dividing layer of cells that lies between and gives rise to the secondary xylem and phloem [1- 3]. Wood is formed through cambial activity, promoting growth and cell division in plants’ root, stem, and leaves [4-6]. The multiplication and division of these cells cause plant girth to increase and stimulate the production of xylem and phloem cells. Nutrients and water uptake are regulated by xylem tissue inside the vascular cambium [7, 8].
In comparison, sugar and other macromolecules are transported by phloem tissue outside the vascular cambium. In woody plants, secondary cork produced by cork cambial cells is composed of a thick viscous substance that might have hydrophobic activity. The bark is the outermost layer of woody trees formed by cork cells, which protect plants from physical damage and environmental stresses and reduce water loss [9-11].
The structure and function of the vascular cambium provide information on genetic components and the mechanisms underlying the secondary growth of plants. Modern molecular approaches can modify the cambial structure to produce a dynamic population of plant cells. Therefore, to identify the mechanisms that determine which cells serve as cambial stem cells, it is important to find how the fate of these cells is sustained, the patterning of vascular tissue involved in the fate of xylem from phloem cells, and how equilibrium is maintained in stem cells compared to the differentiation of newly formed cells [3]. Many environmental factors (including temperature, humidity, and photoperiod) affect plant cells’ internal cell structure and development [12, 13]. The direction of cambial formation is unclear in the initial stage but becomes uniform in the final stage. However, there is no clear evidence of the direction and arrangement of cambial cells. When the vascular cambium reaches the dormancy stage, growth is initially retarded at the basal part of the tree, followed by the uppermost part [14, 15].
Variations strongly influence the mechanism of xylogenesis in plants in temperature, sudden rainfall, and other climatic factors. Cambial cells remain more active under high water levels longer but are more sensitive [16, 17]. Another recent study showed that temperature, environmental variation, and time influence of cambial activity in Qilian Juniper. This study found that, during spring, cambial activity was upregulated with increasing day length and was not influenced by water availability. However, during late summer, cambial latency was down-regulated in plants flooded with water. It was highly stimulated in underwater plants, limiting regulated conditions by reducing day length [18].
The molecular mechanism underlying the effects of different environmental stresses on cambial activity is complex and still requires clarification.
Many soils in the world contain inadequate phosphorus (P) in inorganic P accessible for plant development; however, P is rarely present in soil solution compared to other macro and micronutrients [19-22]. The distribution of P into the soil is heavily controlled by plants, contributing to the emergence of P-depletion areas. In different plant species, the amount of P increased the volume of the stem by increasing the proportion of the large diameter. However, it lowered the density of wood [23]. Root elongation is extremely sensitive to the environment. Consequently, when such spatial and temporal changes occur, P, nitrogen (N), and iron (Fe) affect root development.
Review studies on stem and root cambial activity subjected to different environmental and nutritional disturbance types. Specifically, this review focuses on the physiology, anatomy, regulation of cambial reactivation, and xylem differentiation across different plant species, as it concerns the quality and quantity regulation and the adaptability of plants to the environment. Different regions in the globe contain insufficient P, and plants in the soil severely controlled P for better growth and development. That is why we studied the effect of phosphorus, temperature, and water stress on cambial activity.
Cambial Activity in Response to Temperature Stress
The timing of cambial reactivation contributes to determining the amount and quality of wood produced and showing the environmental adaptability of trees. Environmental factors, like temperature, have a major effect on the development of the tree stem [3, 24]. Temperature affects the physiological development of the vascular cambium, including the onset of cambial cell division and xylem differentiation in trees from late winter to early spring. During this period, cumulative high temperature leads to the earlier onset of cambial reactivation and xylem differentiation in trees and facilitates a continued growth period. Cold tolerance reduces after cambial reactivation because earlier cambial reactivation may increase the risk of frost damage [25]. Several studies have demonstrated that temperature controls the timing of cambial reactivation, affecting the quantity and quality of wood [26-28]. Earlywood thickness and area of earlywood vessels in Quercus crispula have risen due to the long-term temperature increase in the early spring, which influenced the timing of the beginning of cambial reactivation in winter dormancy [29]. Increasing temperature trends have led to early cambial resumptions extending the xylogenesis period and prolonging the growth of more xylem cells [30]. The tree-ring structure, widely researched in ecological studies, permanently shows the environmental regulation of wood formation [31]. Temperatures in late winter and early spring give significant external stimulation to induce the changes in C. japonica and hybrid poplar and xylem distinguishing in the temperate area [32]. In another study, over a particular threshold value of the mean daily temperature of 5.6 to 8.5ºC, the cambial activity and xylem differentiation happened in three conifers species (Larix decidua, Pinus cembra, and Picea abies) [33]. The minimum air temperature threshold for the xylem differentiation onset in Rhododendron aganniphum was 2.0±0.6ºC [34]. Therefore, the temperature seems to differ between different species [5]. Conclusively, the temperature is a key operator of xylogenesis at the onset of the growing season in cold climate zones. As global warming continues, consequently, the beginning of xylogenesis may be thought to happen earlier in the year [35, 36].
The vascular cambium is situated between the secondary xylem and phloem, which develop during the early growing period. Throughout the inactive stage, it comprises two or three layers of cells, which are radially compacted and narrow in absorbent diffuse hybrid poplar (Populus sieboldii × Populus grandidentata). New cell plates develop in the vascular cambium from late winter to early spring, termed the cambial reactivation phase [37]. Cambial reactivation has been examined in Citrus limon [38]. The electron microscope is normally used to identify the internal structure and variation in cambial cells through natural reactivation and cytoplasmic differentiation accompanying the onset of cambial cells. It also examines different species’ structural changes between dormant and reactivated vascular cambium. An electron microscope was operated to detect the measures happening in the cambial zone, and definite information regarding the role of individual cambial cells was obtained during the reactivation period [39].
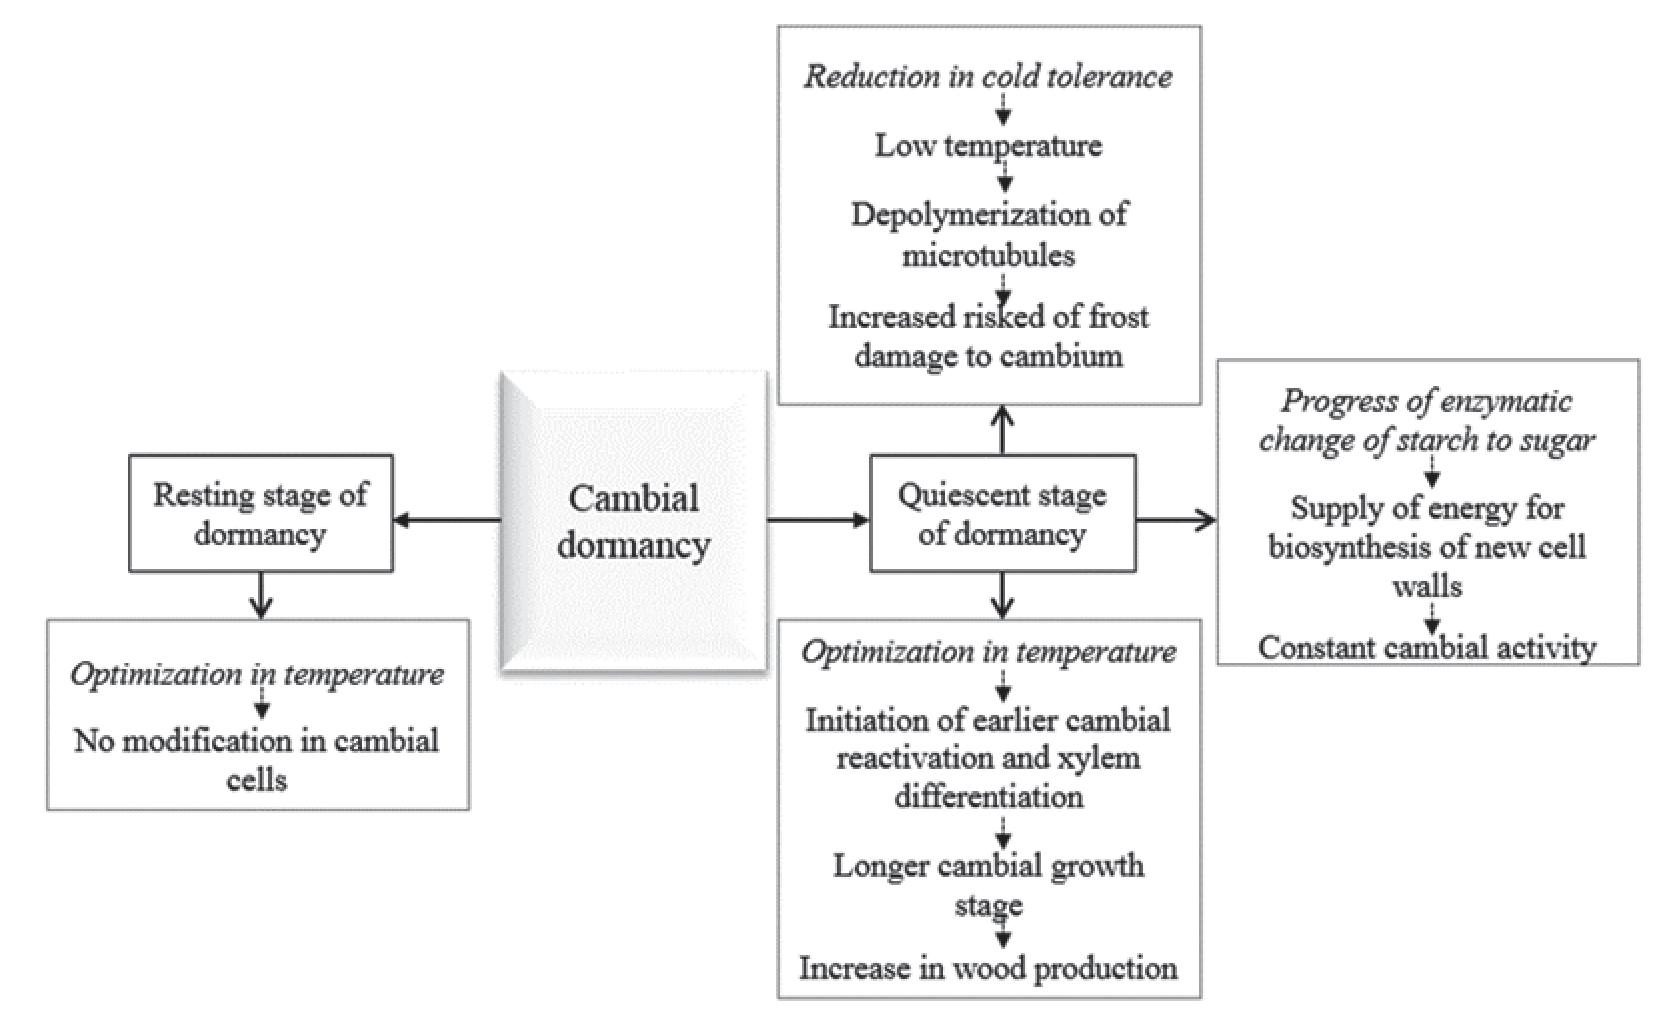
Cambial activity can last all year in a tropical climate, whereas cambial activity in a temperate climate is usually seasonal [40]. Therefore, photoperiod is an essential factor affecting cambial activity in plants [14]. Temperature is one of the most critical environmental elements that impact plant growth, where late winter to early spring greatly influences cambial cell division and xylem differentiation. The cumulative effect of temperature causes cambial reactivation, and xylem differentiation in plant stems begins earlier than usual, extends the growth phase, and increases the risk of frost damage [26, 32]. When meristematic activity stops, a dormant phase begins and continues until the cell division cycle is restarted [41, 98]. Winter cambial dormancy has two phases: (i) the resting phase that is governed by endogenous causes; (ii) there is also quiescence dormancy that is influenced by exogenous factors [42]. There are structural, functional, and histochemical changes to cambial cells from the resting to quiescence stages [14, 32]. Even in favorable circumstances, when indole-3-acetic acid (IAA3) is applied, the cambium cannot generate new cells over the first 2-4 weeks of dormancy in the resting phase [43]. After artificial or natural chilling, the cambium’s ability to produce new xylem cells progressively improves in response to IAA under a favorable environment. This stage is referred to as the quiescent stage. The complete responsibility of the cambium to IAA is facilitated by conflicting external factors [44]. Endogenous IAA was observed in the cambial zone of the conifer Larix kaempferi and hardwood Quercus rubur [45]. In dormant quiescent, the endogenous IAA levels can be sufficient for maintaining and reactivating the cambial cells and distinguishing the initial vessel elements [46]. Moreover, this change between the two phases varies substantially between different species. About dormancy and cambial activity, the most commonly used terminology is shown in (Fig. 1).
The reactivation of the vascular cambium in Abies sachalinensis and Picea abies was stimulated by the calcification of stems at 23ºC to 27ºC and 24ºC to 30ºC for five to six days, respectively, during winter [27]. Consequently, throughout the quiescent dormancy of trees, an increase in temperature might limit the onset of cambial reactivation. In a deciduous diffuse-porous hybrid poplar, P. sieboldii × P. grandidentata, the confined heating of the tree stem facilitated the division of phloem parenchyma cells during dormancy [47]. The timing in the cambial reactivation of heated and non-heated control portions of tree stems differed by almost four weeks. Four weeks of confined heating facilitated the reactivation of the vascular cambium, which happened earlier than the reactivation under natural conditions. Thus, in winter, the response of cambial reactivation to heat treatment might be useful for studying the dynamics of cambial reactivation because it is easy to activate the division of phloem parenchyma cells and promote secondary xylem growth from cambial cells. Cambial reactivation directly occurs by increasing the temperature of tree stems [48]. However, the later onset of cambial reactivation is associated with a sudden decrease in temperature. Late spring frost might cause the cold tolerance of the vascular cambium to decline, which is facilitated by the depolymerization of microtubules and negatively influences tree development. The timing of cambial reactivation is associated with cambial age. Under heated and natural conditions, cambial reactivation and xylem differentiation happen earlier in 55-year-old cambium compared to 80-year-old cambium [26]. The cambial mechanism differs between young and old trees, even when grown under the same environmental conditions. Thus, the cambial response to temperature might be associated with the age of vascular cambium in Pinus pinaster stems [49].
Cambial Activity in Response to Water Stress
The xylem developmental process is defined by five consecutive differentiation stages: cell division, enlargement, cell wall thickening, lignification, and programmed cell death. Xylem cell anatomy is influenced by different climatic conditions (water availability, temperature, nutrients, and genetic predilection), with the anatomical features of intra-annual cell sequences potentially providing seasonal climatic information [50-52]. For example, the phases of cell enlargement are impacted when several vacuoles cumulate into one large central vacuole, which receives more water. During this stage, the enlarged tracheids achieve their last radial diameter, and the water supply level, therefore, regulates the size of the cell dimension of the radial [53, 54].
Fig. 1.
Schematic outline of annual stages of dormancy and cambium activity. Resting stage cause temperature optimization results in no cambial cells modification. Quiescent stage reduces the cold tolerance that increase frost risk for cambial damage while optimising the temperature for cambial growth. The effects of rising temperatures from late winter to early spring on wood development in trees [14, 32].
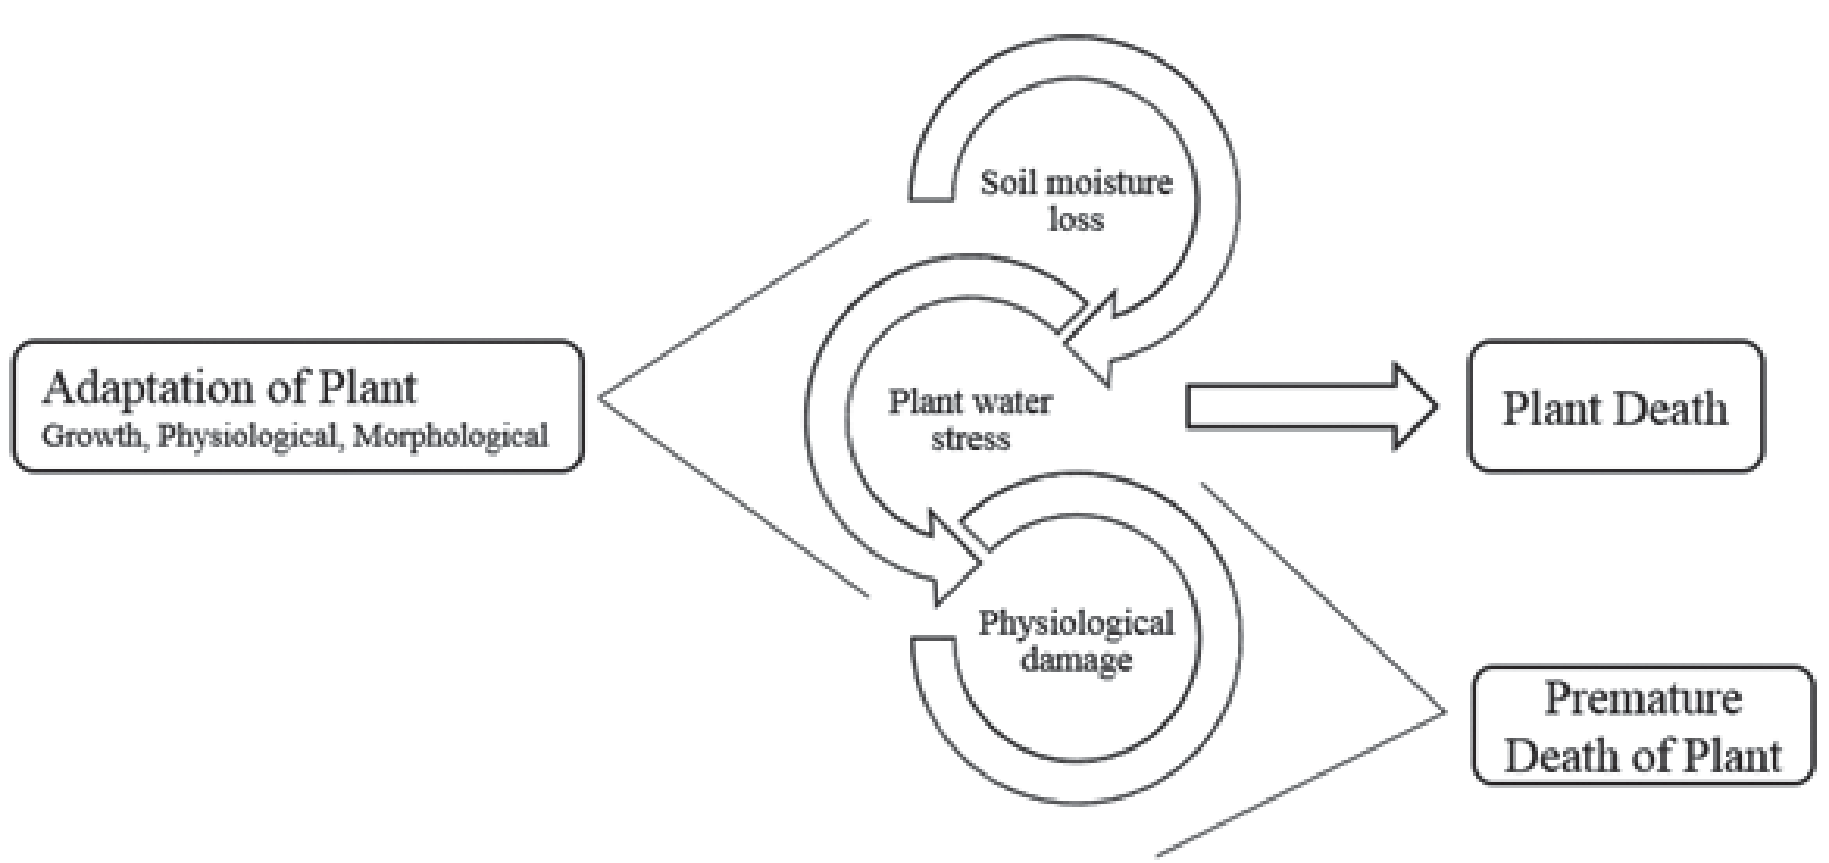
Certain western Mediterranean basin areas are characterized by cold and wet winters and hot and dry summers. Consequently, cambial activity might be subjected to two types of disruptions: (1) low temperature in winter and (2) high temperature in summer, which causes water stress [55]. Diverse seasonal patterns of secondary growth might occur, depending on the autecology of species and different climatic conditions each year. Thus, the anatomical physiognomies of wood cells might be affected by climatic conditions and the autecology of the plant species [56]. Water stress, directly and indirectly, affects Xylem growth [57, 100]. Cell enlargement is substantially inhibited by damage caused by cell turgor due to water scarcity at the early stage [58]. Stress affects the physiology of the entire plant and inhibits cell metabolism; ultimately [59], the growth becomes retarded as the water scarcity remains (Fig. 2) [60]. In another study, ray cambial cells and fusiform cells facilitate continued turgor when applying adequate water stress (Ψx≥P50) to plant seedlings. However, fusiform cambial cells dehydrate and lose turgor (i.e., Ψx≤P50). Plants with -3.7 MPa water stress exhibited less cambial damage, while plants with –3.2 MPa exhibited severe cambial damage. Thus, plants might exhibit individual responses to drought by varying the vascular cambium structure [61, 62]. The drought that has regularly happened in temperate forests over the last few decades is now viewed as a global problem that can considerably impact the forest cover over large regions. During the growth season, periodic changes in the cambial activity are responsible for variations in earlywood and latewood areas from the “regular” succession [63-65]. The prevalence of variations of intra-annual density was mostly investigated in Mediterranean habitats, while it was also found in other environmentally induced ecosystems (e.g., temperate, tropical, and boreal ecosystems) [66-67]. Drought inhibits the physiological function of trees, leading to dieback and fatality. Scots pine trees are found in drought by decreasing the tracheid’s number and cell wall thickness and consistently developing its lumen diameter, minimizing the carbon costs of their water conduction system [68-70]. Examining the dimension of xylem cells can provide valuable information for the behavior of the tree during intense droughts.
The amount and time of cambial production affect the annual radial increase in trees. Cambial cell divisions are responsible for developing new xylem and phloem elements, directly affecting water transportation efficiency, mineral nutrients, and photoassimilates [71]. Consequently, the new cells are controlled by fluctuating cambial phenology [72]. Drought stress variation and long-lasting lack of precipitation associated with thermal waves significantly changed cambial temperature. Cambial cell divisions were observed to be reduced when the average air temperature was above 25ºC, the potential soil water values decreased below −1MPa, and fewer changes were seen [73]. According to the studies, during the last week of July, the number of cambial cells started to rise in the environment of abundant rainfall following the June shortage in 2014. In conclusion, the number of produced tracheids and their radial diameters decreases comparatively, increasing the hydraulic efficiency of Scots pines suffering water stress.
Fig. 2.
A simplified diagram demonstrated the water stress on plant growth, morphology, and physiology. Premature death of a plant happens due to water stress conditions [60]. The growth response of a Mediterranean tree species, Juniperus thurifera, specifically declined due to comparatively dry and warm summers [62, 63]. Thus, in Mediterranean areas, cambial activity depends on water availability throughout the growing season [64]. By increasing water stress, stomatal conductance decreases [65, 66]. When stomatal conductance was <110 mmol H2O•m–2•s–1, the author’s perceived radial development termination [67], underwater stress, and cambial activity decline and adversely affect xylem production [68,69]. The stomatal conductance is reduced within eight days, while radial growth stops within twelve days after water scarcity starts [67].
Cambial Activity in Response to Phosphorus Stress
The physiological function and the economic value of tree stems are affected by wood density [74]. Therefore, modifications in wood density must occur due to differences in the overall proportions of cell walls and lumen. In contrast, wood density is affected by the extractable substances in the cell wall material [75, 76]. In Pinus radiata, the amount of phosphorus increased the volume of the stem by increasing the proportion of the large diameter; however, it lowered the density of wood [77]. P supply influenced the density of Eucalyptus grandis seedlings by the biomass segregation of the stem rather than by modifying biomass partitioning of the entire plant. With the reduction of the P supply, the biomass segregated towards the stem was preferably employed to thicken secondary fibre cell walls rather than to produce more cells. Due to the independent P supply from fibre cell diameter, increased fibre wall thickness was primarily responsible for developing wood densities [78, 79]. Low P availability encouraged the fibre cell’s secondary cell wall thickening. This resulted from a decrease in the development of new fibre cells.
The stem diameter with decreased P supply was reduced by 80 percent, which caused a reduction in the cell population since the cell diameter remained constant [78]. Wood stem cells compete dynamically for photoassimilates, and this competition intensifies as the cambial zone of the stem becomes more active [80]. As evidenced by the fibre cell numbers, the cambial activity of the stem was significantly more reliant on P supply, unlike secondary wall thickening. Therefore, more assimilates are accessible for the secondary wall thickening when the P supply restricts the cambial activity. The seedlings’ height, stem diameter, and volume improved as the supply of P increased. However, wood density and stem anatomy were resistant to the provision of high P. The consistency of the wood density at the high P level is characterized by the fi-ber-cell-anatomy under a high P level. The biomass provided to stems under high P levels was intended to promote cell multiplication instead of enhancing existing cell wall synthesis [78].
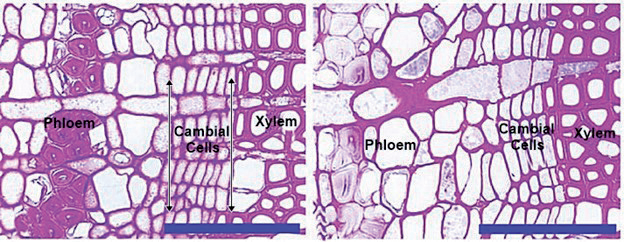
Cambial mechanisms have been defined in the shoot apical and root apical meristem under different environmental and nutritional disturbances, with most studies examining the stem and root together. The activity of the vascular cambium was significantly affected by different environmental stress conditions. The growth of cambial cells was observed as immature, they were diffused with each other at the initial stage, and the direction of cambial formation was not very evident. The cambial cells gradually became uniform with the passage of time at the final stage (Fig. 3). The number of cambial cells showed an apparent expansion of the cell enlargement process at the time of maximum cambial activity.
The root is a sensitive portion of a plant exposed to the soil environment; thus, it is important to understand how the vascular cambium performs its functions in the root system separately and clearly. Cambial activity is the most important factor for understanding the mechanism of the root system under different environmental stresses. However, knowledge of cell physiology, specifically cambial activity, remains inadequate for interpreting information in the root system of different tree species. To enhance predictions, how different environmental stresses influence the activity of the cambium, particularly concerning mechanisms in the root portion of trees, studies need to focus on establishing the mechanisms of xylogenesis using endogenic and exogenic approaches. This approach might represent a novel method for establishing timber quality in production and for other medicinal purposes.
The root systems of different plant species contribute to water and nutrient uptake and anchoring of the soil and are essential for establishing biotic relations in the rhizosphere [81]. Several processes affect cell division and elongation rates, lateral root growth, and root hair growth [82]. Root elongation is extremely sensitive to the environment. Therefore, during spatial and terrestrial changes, phosphorus, nitrogen, and iron alter root development. Thus, soil nutrients change the structuring of roots through specific signal transduction pathways [23, 83].
Many soils in the world contain inadequate P in inorganic P accessible for plant development; however, compared to other mi-cro-molar elements, P is rarely present in soil solution [21]. The distribution of P into the soil is heavily controlled by plants, contributing to the emergence of P-depletion areas. Because of the restricted availability and slow motion of soil P, the increase in soil volume by the root system is one of the most effective ways of improving P uptake. That is why the root shoot ratio under P stress is increasing [23, 84]. While improving the allocation of resources for root growth increases P acquisition, uneven root growth affects total plant growth since the addition of the root tissue would increase the metabolic cost [82, 85, 86]. This cost focuses on three components: new root tissue growth, ion absorption, synthesis, and current root tissue preservation [82, 87]. As a result, moderating maintenance expenses are the biggest potential to minimize the root system metabolic burden.
Under P stress, enhancing metabolic productivity is assumed to be an adaptive strategy under which primary growth (elongation) becomes greater than secondary growth (radial thickening) in the root system to explore the surrounding soil [19]. Studies of the root system under P stress have identified the importance of root diameter in different plant species [88]. The diameter of the roots of the sedge Carex coriacea declined by 30% from high P to low P; thus, root length is negatively correlated with P availability [89]. In another study of temperate pasture species, the root mass density and root diameter declined under P stress while the root length increased [90, 91]. However, whether root diameter declines under P stress for all root categories is unknown, with the results of current studies potentially being associated with higher-order lateral roots rather than the effects of improved secondary growth. Specific studies on secondary growth within root classes are required under P to determine whether the decline of secondary growth is an adaptive response [92]. During secondary growth, the periclinal splitting of cells and separation of secondary tissues at the vascular cambium cause major destruction to the cortex, epidermis, and endodermis. Although the production of periderm changes primary tissues and protects root vasculature, thickening during secondary growth is determined by the results of secondary xylem elements and parenchyma [93]. The exclusion of the primary tissue and an increase in secondary tissue have been observed in transverse divisions. These phenomena occur through the loss of cortex, epidermis, and endodermis, parallel to an escalation in the number and size of meta-xylem vessels and the enlargement of the stele. For plants under P deficiency, root anatomy changes regarding stele diameter, root diameter, and meta-xylem vessels, along with smaller and fewer epidermal cells, xylem vessels, cortical cells, and a smaller percentage of stele parts [94, 95].
Fig. 3.
Differentiation between cambial cells, xylem cells and phloem cells. A transverse view of cambium in light micrographs in which cambial cells are compactly organized between the phloem cells and thick-walled xylem cells. The cambial cells were identified individually by considering all cells having a thin wall and a small radial diameter [25].
Discussion
Many studies have investigated cambial growth and xylem formation in the stem and roots directly associated with xylogenesis. These studies identified changes in cambial activity, xylem formation, cell differentiation, and differences in production between the stem and the roots. Xylem production in the stem occurs early in the season, whereas differentiation in root cells occurs one month later. Similar cell differentiation phases occur in the xylem in both the stem and roots, yet intra-annual growth dynamics vary [3, 96-98].
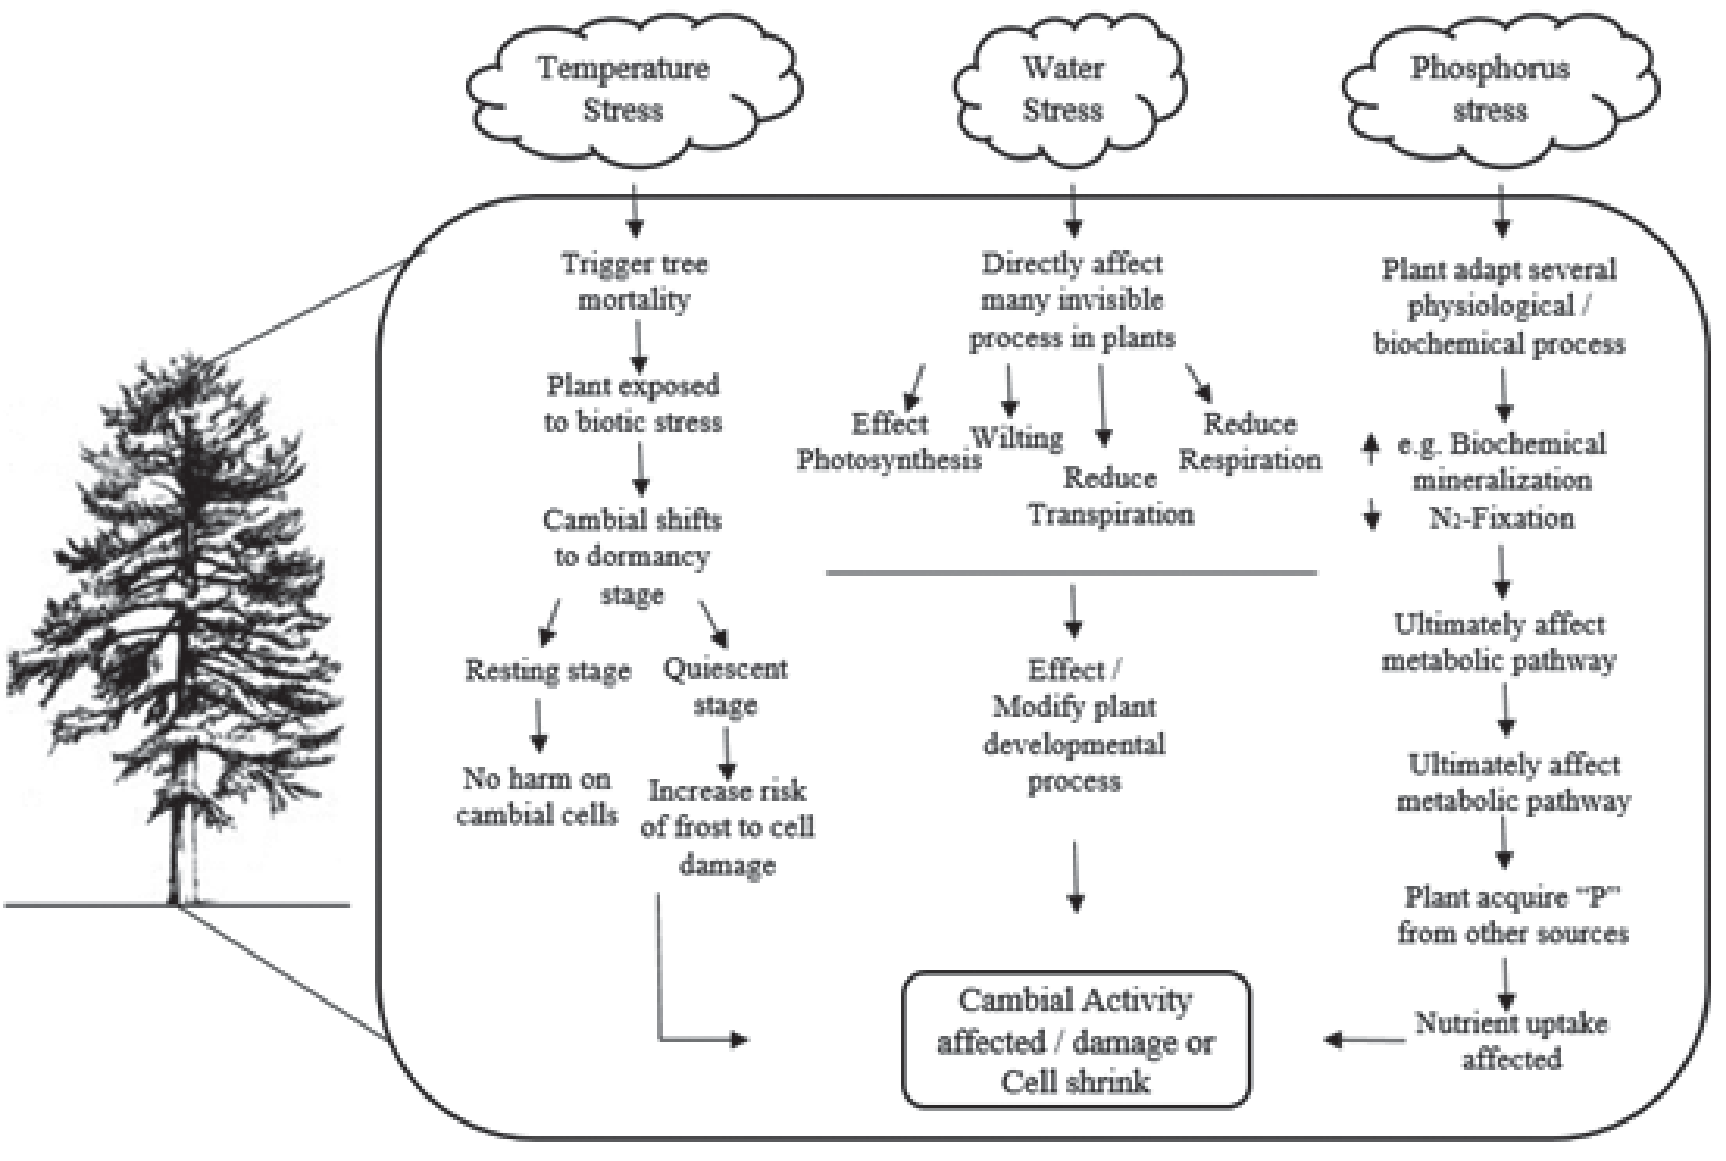
Environmental and stress conditions are the primary targets of mobile signals that modulate cambial cell activity [99-101]. This phenomenon might be associated with internal and external factors, including the number of cells produced by the vascular cambium and various configurations of soil temperature and air during spring. Another study predicted that higher temperature might be reactivated the cambial cells and consequently the development of phloem and xylem cells, but low water availability may change the time of cambial cell initiation, which may cause the formation of vascular tissue narrow due to reducing capacity of xylem-driven water transport [102]. Transpiration stream is critical due to the formation of vascular tissue, which might be in appropriate formation, along with entire photosynthesis [103]. Different environmental and physiological parameters influence cambial activity and, hence, the development of meristems (Fig. 4). The influence of both modulators, high temperature, and seasonal change directly affected the relationship between the start of xylem differentiation and induction of cambial reactivation [104]. Variations in climate responses could cause a change in cambial activity. Drought can prevent the phenomena of turgor-driven cell growth and reduce cambial cell division [105]. Auxins regulate genetic variation in the xylem, forming a concentration slope over evolving tissues and forming a crown around the vascular cambium. During the process of xylogenesis, the cambial zone might represent a significant carbon sink. Thus, the energy required for metabolic processes regulates cambial cell division and the end products of cambial cells [26]. During cell differentiation, three key phenological phases (onset of growth, maximum growth, and completion) are strongly influenced by environmental factors, such as photoperiod and temperature [24,106]. During these stages of growth, more knowledge about the availability of carbohydrates is required to elucidate stem growth mechanisms. At the beginning of cambial cell division and xylem differentiation, temperature influences physiological development from late winter to early spring [14]. An overall rise in temperature from late winter to early spring causes the early initiation of xylem differentiation and prolongs the growth phase. However, earlier cambial reactivation increases the effect of frost damage due to a decline in cold tolerance after cambial reactivation. By rising temperature, the sensitivity of specific species may be narrowly correlated to the temperature of cambium and its changes from a dormant to an active state [107].
Fig. 4.
A representative diagram exhibited different environmental factors, like temperature stress, water stress and phosphorus stress effects on the cambial mechanism in plants [32, 61, and 95].
It has been hypothesized that this phenomenon is an adaptive strategy to improve the metabolic efficiency of soil foraging under P stress. For instance, roots might favor primary growth (elongation) over secondary growth (radial thickening) to explore a greater area of soil to locate areas that have not been depleted of P [82]. In a study of the root morphology of temperate pasture species, reduced root diameter and root mass density, in parallel to increased specific root length, were observed under P stress [90, 108]. Secondary growth eliminated eradicated mycorrhizal associations as cortical tissue was destroyed. This is a supportive statement that reduced root secondary growth is an adaptive response to low phosphorus availability for potential breeding targets [109]. Observations of how root diameter reduces under P stress across root classes have not been quantified. Thus, reductions to the root diameter of the entire root system might be the product of a greater proportion of higher-order lateral roots rather than the effects of altered secondary growth [82, 106]. Under P deficiency, observed changes to the root anatomy of a variety of species included smaller root diameter and stele diameter, fewer and smaller epidermal cells, and meta-xylem vessels, a reduced percentage area of stele coverage, and fewer cortical cells and xylem vessels [94, 110]. Further work is required to determine the influence of reduced metal conductance in roots with reduced secondary growth on metal capture in soils. In particular, targeted studies are required on the relationships between secondary growth and the colonization of different tree species.
Here, reviewed the cambial mechanism under different levels of drought stress [96, 111]. Ultra-structural modifications in the cambial structure likely provide morphological and hydraulic indications of water stress responses in plants at the cellular stage. This review also highlights the water stress responses of rooted cuttings cultured at a cambial level under hydroponic conditions, e.g., [61, 112].
Under this technique, the nutrient solution level can be reduced at different speeds and could be used to examine the adaptative and non-adaptative drought responses of cambial tissue involved in wood formation under restricted water availability. This approach represents a competent model for studying cambial activity and wood formation. This review also showed that temperature, water, and phosphorus dynamics indicate past and current functions of different tree species [113]. In particular, this review demonstrates the need to research mechanisms within a classified scheme and how identified stresses vary in relation to the physiological and morphological features of different tree species over specific periods.
Conclusion
To understand the literature on the effects of environmental and nutritional stress on stem and root cambial activity, this review focuses on the physiological and anatomical differences across varieties of plants, as well as the regulation of cambial reactivation and xylem differentiation because these factors affect plant quality and quantity regulation and adaptation. Conclusively, an increment in stem temperature caused by environmental influences could directly cause the breakage of cambial dormancy in trees, but the responses to certain changes in temperature varied between different species based on the dormancy stage. The temperature rises from late winter through early spring could lead to earlier cambial reactivation and differentiation of the xylem, leading to prolonged periods of fluctuating growth and increased wood biomass production. An abrupt reduction in temperature after the onset of the cambial reactivation, including a late-spring frost when the cambium’s cold tolerance is inadequate, could promote microtubule depolymerization, with a subsequent negative influence on tree development and growth. Significant responses from the changes to drought stress have been discovered in this investigation. Drought stress started to decline the quantity and radial dimensions of produced tracheids to enhance hydraulic activity. Low P restricted stem cambial cell activity, enhancing the number of photoassimilates available for secondary fibre cell growth and, consequently, the wood density of different plant seedlings.

