

Introduction
Wheat (Triticum aestivum L.), a major cereal crop, is constrained by drought in numerous regions of the world. Because of severe limitations imposed by drought, the development of cultivars with improved productivity under water stress is important for affected regions. However, the development of drought-tolerant cultivars is hindered by a lack of understanding of the mechanisms of drought resistance and reliable selection techniques. Because wheat production in our country is mainly dependent on precipita-tion conditions, it can show significant fluctuations from year to year. In some years, especially with insufficient rain-fall, wheat production decreases considerably. As a result, some consider drought as the main environmental stress for different plants, particularly in drought-prone areas [1], the single most critical threat to world food security in the future and the catalyst of important famines in the past [2]. Plant drought-stress tolerance, the ability of plants to maintain productivity during periods of drought stress, is a complex phenotype [3]. The decrease in productivity under drought stress conditions is one of the most important factors threatening global food production [4].
Plant drought-stress tolerance, the ability of plants to maintain productivity during periods of drought stress, is a complex phenotype [5]. Plants have numerous mechanisms to tolerate drought stress at the organ system to cellular levels, including adaptations in plant growth and development, resulting in alterations in plant allometry, root system development, and even time to flowering, osmotic adjustment, and optimization of water use [6]. The mor-phological and physiological responses of crops to drought can explain the large variation in yield under drought stress conditions [7].
Drought stress causes a number of biochemical, mor-phophysiological, and anatomical disturbances in plants that occur at all stages of plant development, from seed germination to the final stages of the generative phase [8]. Drought tolerance in plants is the result of numerous inter-related mechanisms that operate at the molecular, cellular, and organismal levels. Among them are changes in the state of the stomatal apparatus, and accumulation of various osmolytes in cells [9, 10]. The maximum quantum yield of primary photochemistry in leaves in the dark-adapted state can reflect wheat’s light-use efficiency under drought conditions [11]. The relatively low canopy temperature value at the grain-filling stage and the high chlorophyll content during the late grain-filling stage can be used to screen the winter wheat cultivars adapted to dryland eco-systems [12].
Wheat is very sensitive to drought during the early seedling stages and germination. Insufficient available water in the early development stages significantly constrains grain yield through decreasing germination, emergence, and seedling development and establishment [13]. Seedlings of plants are extremely sensitive to drought stress conditions [14]. Drought stress affects water balance, disrupts meta-bolic reactions at the cellular level, reduces ATP synthesis and respiration, and results in poor seed germination [15].
The aim of the study is to reveal the effectiveness of the survival ratio, canopy temperature, chlorophyll content, and stomatal characteristics of the seedlings after experiencing drought conditions in the differentiation of drought-resistant genotypes of 45 genotypes in different seedling mortality ratios.
Material and Methods
In the study, 45 genotypes of different origins, including 39 bread wheat, 1 rye, 1 Spelta, 2 Kavlıca, and 2 Siyez populations, were used as materials. The genotypes used as material in the experiment are given in Table 1.
The experiment was performed in a covered crate environment in order to determine the early drought resistance levels of 45 genotypes used as material in the experiment. Seedling survival level, seedling development score, canopy temperature, chlorophyll content, stomata density, stomata width, and length were examined.
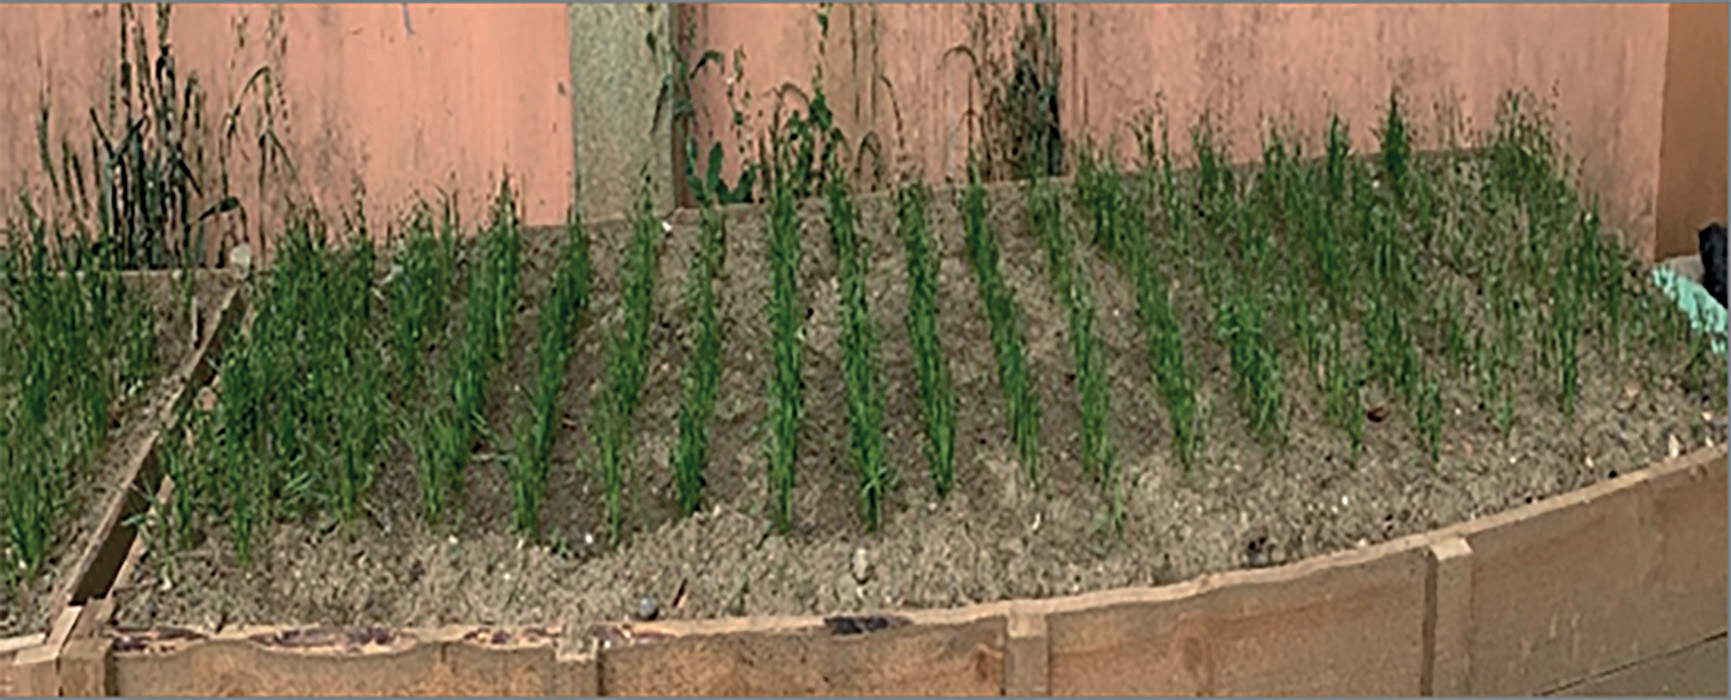
In order to determine the seedling survival level in the experiment, a 10-meter-long and 1.2-meter-wide crate was constructed (Fig. 1). Table 1 cont. Genotypes used as material in the experiment
Table 1.
Genotypes used as material in the experiment
Soil samples taken from Tekirdag Namık Kemal University, Faculty of Agriculture, Department of Field Crops trial area were filled into the crate with a depth of 20 cm and water was given until the soil was saturated. According to the soil analysis taken from the trial area, the soil has a pH close to neutral, a loamy soil structure, and low organic matter (1.03%). When the soil was at the right level, each genotype was sown with a length of 1 meter and 1-row spacing (26.05.2021), and 500 seeds were used per square meter. Irrigation was applied until the plants had 3 leaves (07.06.2021), and then no irrigation was applied until it appeared that more than 90% of the seedlings died due to lack of water (27.07.2021).
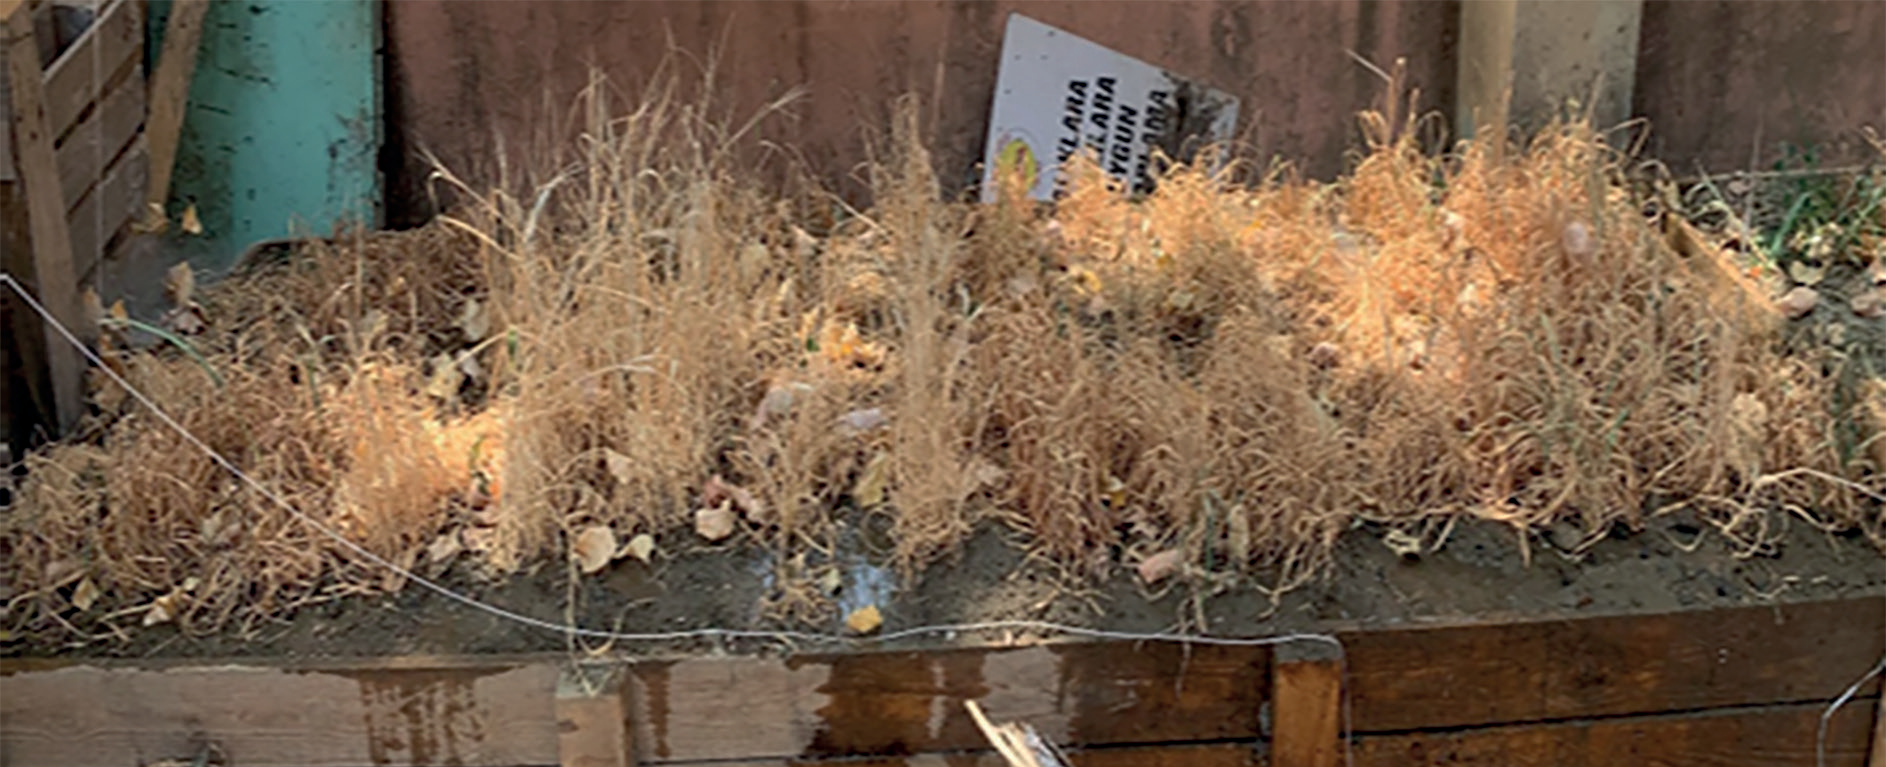
Plants were subjected to 50 days of drought stress, and when it appeared that most of the plants died due to the lack of water (27.07.2021), irrigation water was given to the crates. Irrigation was repeated at regular in-tervals and seedling survival ratios were determined again (22.08.2021). Seedling survival after drought was calculat-ed as a percentage [16]. The plants were given a score of 1 for no plant development, 2 for plant development between 1–5%, 3 for plant development between 5.1–10.0%, 4 for plant development between 10.1–15.0%, and 5 for plant development exceeding 15% (Fig. 2).
The canopy temperature, chlorophyll content, stomata density, width, and length characteristics of the plants developed at the beginning of the formation of stress images were determined. The chlorophyll content of flag leaves on the main stem of plants was measured with a “Konica Mi-nolta SPAD-502” portable chlorophyll meter. The canopy temperature was determined with an infrared thermometer. Analysis of variance was performed on the data obtained and the Tukey (P < 0.01) test was used to determine the differences between genotypes.
Results and Discussion
The seedling development scores of 45 genotypes sown in the rows in the crate environment are given in Table 2. As seen in the table, seedling development scores varied between 1 and 4. The scores of Adelaide, Başkan, Refikbey, Spelta, Kavlıca color, and Siyez 2 genotypes were the lowest with a score of 1. In terms of seedling development, 15 genotypes in the experiment had a score of 2 while 16 genotypes had a score of 3. Among the genotypes included in the experiment, Maden, Enola, Mihelca, Maya, Ambrosia, Hamza, Aglika, Anapo and LG 59 had a score of 4 for seedling development. According to the data, it was determined that varieties in the early and mid-ripening group, such as Hamza, Aglika, Anopa, and LG 59, had higher seedling development scores [17].
When the survival ratios of the seedlings were evaluated again after the drought in the genotypes included in the experiment, no seedling survivability was observed again in the Adelaide, Başkan, Selimiye, Hakan, Quality, Hamza, LG 59, Golia, Siyez 1, and Siyez 2 genotypes. TT 601, NKU Lider, NKU Ergene, İveta, Maya, Ambrosia, and Kavlıca white genotypes had a score of 2 with seedling survivability between 1–5%. Prima, Anica, Mihelca, Bora, Pannonia, Masaccio, Sarı Mustafa, Refikbey, Spelta, and Kavlıca color had a score of 3 with seedling survivability between 5.1–10.0%. NKU Asiya, Maden, Enola, Bezostaja 1, Energo, Misia Odes’ka, Aglika, Kaan, Genesi, and Ducato genotypes had a score of 4 with seedling survivability between 10.1–15.0%. Esperia, Rumeli, Krasunia Odes’ka, Almeria, Falado, and Rebelde had a score of 5 with seedling survivability ratio of more than 15% (Table 3). The mor-phological and physiological responses of crops to drought can explain the large variation in yield under drought stress conditions [18]. In the study, seedling weight, root number, root length, root weight, shoot length, and shoot weight characters were determined. It was determined that drought stress applications caused statistically significant decreases in root and shoot characters. Osmotic stress of 1.00 MPa and 0.75 MPa caused statistically significant reductions in root and shoot characters [19].
Table 2.
Seedling development score in the genotypes
Table 3.
Seedling survivability score in the genotypes
None of the genotypes with the lowest and highest seedling development scores were among the genotypes showing the highest seedling survivability (Esperia 2, Rumeli 3, Krasunia Odes’ka 3, Almeria 3, Falado 2, and Rebelde 2). With the obtained data, it was conclud-ed that there was no significant relationship between seedling growth score and seedling survivability ratios. A genotype with drought stress tolerance capabilities has a more developed root structure to reduce the pronounced effects of drought by using soil moisture during development and growth. Various methods were investigated to determine wheat genotypes that are drought-resistant in the seedling period. Selection of wheat varieties on the basis of seedling traits is easy, inexpensive, and less laborious. Similarly, seedling attributes expose moderate-to-high variability with an additive gene effect across environments [20]. It was determined that effective results were obtained in terms of drought resistance by using seedling characteristics and that the material determined for drought resistance in the seedling period could be successfully used in breeding studies [21].
In the analysis of variance performed on canopy temperature, chlorophyll content, and stomatal characteristics of 45 genotypes used in the study, the differences between genotypes were found to be statistically significant and the results of the significance test performed to reveal the differences between genotypes are given in Table 4. Table 4 cont. Significance groups in canopy temperature, chlorophyll content and stomatal characteristics
Table 4.
Significance groups in canopy temperature, chlorophyll content and stomatal characteristics
According to the average values, the canopy temperature varied between 38.67–23.67°C in 45 genotypes. Among the genotypes in the study, the lowest canopy temperature was in Falado cultivar with 23.67°C, followed by Ducato and Aldane with 24.33°C, Iveta with 24.67°C, TT 601 and Maya with 25.00°C, and Almeria and Rebelde with 25.33°C. The highest canopy temperature was 38.67°C in Başkan cultivar, followed by the genotypes such as Adelaide with 36.45°C, Golia with 33.67°C, Siyez 1 with 33.67°C, Spelta with 32.67°C, NKU Asiya with 31.67°C, Kavlıca white and Kavlıca color with 31.33°C, Siyez 2 with 31.00°C.
When the genotypes were analyzed for chlorophyll content, it varied between 49.03-29.43. The highest chlorophyll content was found in Misiia Odes’ka at 49.03, followed by Aglika, Siyez 2, Mihelca and LG 59 at 41.60, 41.50, 41.24 and 41.03 values. The lowest chlorophyll content was found in Siyez 1 population at 29.43, followed by Selimiye with 29.53 and Prima at 29.63. When the genotypes were analyzed for stomatal characteristics, the stomata density varied between 4.00 and 11.00, stomata width between 6.0 and 14.6 μ and stomata length between 14.0 and 36.0 μ. In crops, recent studies are showing that engineering plants to reduce stomatal number may be an effective tool to improve plant WUE and drought tolerance without yield reductions [22]. While the highest stomata density was 11.00 in Maden cultivar, it was followed by Siyez 1 and Anapo varieties at 10.00. In terms of the stomata density, Misiia Odes’ka and Sarı Mustafa at 9.67 and Kavlıca at 9.33 were ranked next. The lowest stomata density was 4.0 in Prima, 4.33 in Hakan, Hamza, Spelta and Anica cultivars. The lowest stomata density was in Prima cultivar at 4.0, and Hakan, Hamza, Spelta and Anica cultivars at 4.33. Plants’ first physiological response to water scarcity is stomatal closure, which reduces photosynthetic activity by slowing the rate of carbon dioxide entry into mesophyll cells [23].
The highest value for stomata length was found in the Esperia cultivar with 36.0 μ, followed by Spelta and NKU Asiya with 32.0 μ. The least stomata length was found in the Siyez 2 genotype with 14.0 μ, followed by Kavlıca color, Kavlıca white and Sarı Mustafa genotypes with 16.4, and 16.6 μ. The highest value for stomata width was found in the NKU Lider cultivar with 14.6 μ, followed by Falado with 14.4 μ, Maya, Krasunia Odes’ka, Selimiye and Rebelde cultivars with 12.6 μ. The lowest stomata width was found in the NKU Ergene cultivar with 6.0 μ, followed by Siyez 2 population with 6.6 μ and Enola genotypes with 7.6 μ.
The reduction in the length and weight of the hypoco-tyl in seedlings due to water stress can be mitigated with the application of gibberellic acid, which helps to maintain the internal water balance and the protein synthesis in drought stressed plants [24]. Hence, certain genotypes and cultivars, which are drought susceptible and unable to adjust to environmental conditions, resulted in low water-use efficiency [25].
Conclusions
When 45 genotypes in different maturing groups were examined for seedling survivability after drought application, 11 genotypes, including Adelaide, Başkan, Selimiye, Hakan, Quality, Hamza, LG 59, Golia, Siyez 1, and Siyez 2, did not show seedling survivability, while Esperia, Rumeli, Krasunia Odes’ka, Almeria, Falado, and Rebelde were the genotypes that showed the highest seedling survivability with a score of 5. Genotypes with low canopy temperature and high chlorophyll content showed higher seedling survivability. The data obtained show that early seedling survivability can be used in the selection of genotypes for drought resistance.

