

Introduction
Triticum aestivum, commonly known as wheat, is a prominent cereal crop of the Poaceae family [1]. It is an annually cultivated, self-pollinated, long-day plant. Wheat is highly nutritious, containing about 55% carbohydrates, and provides more fiber than any meat-based food [2]. We get our daily energy requirements from proteins, vitamins, and minerals (Mg and P) that come from wheat [3]. Wheat straw is used as animal feed, bedding, compost, and paper rumples. The wheat grain retains fat and mineral matter (1.5-2.0%), sugar (2-3%), fiber (2-2.5%), protein (10-17%), and starch (60-70%). Over the years, wheat yield has increased progressively; however, there is still a gap between wheat demand and yield worldwide [4].
Wheat is cultivated on more than 240 million hectares worldwide, with an average productivity of 2500 kg/ha, which is the highest value at the global level of any other crop [5]. In Pakistan, wheat accounts for 1.7% of GDP and contributes 9.1% of all agricultural yield; however, there is around a 60% yield gap in wheat crops. This huge gap is due to several factors, including late planting of the wheat crop, lack of good-quality seed, improper row spacing and seed rate, poor fertilization, poor irrigation management practices, and weed infestation [6]. Wheat was grown in Pakistan on an area of 8734 thousand hectares in 2017-18, 2.6% less than 8972 thousand hectares during 2016-17. In 2017, 25.492 million tons of wheat were produced, recording a decline of 4.4% over the production of 26.674 million tons the previous year [7].
Several environmental stresses (abiotic and biotic) have decreased per-hectare in wheat production. Due to abiotic and biotic stress, farmers and agriculturalists lose almost 20-70% of their annual crop yield, but upgrading crop yield programs can overcome this loss. Scientists are developing high-yielding wheat varieties and lessening the losses caused by environmental and biotic stresses [8]. Due to limiting restrictions such as water stress, salt, diseases, and the effect of metal toxicity on crops, achieving the predicted goal of yield enhancement is becoming unviable. It requires highly productive wheat varieties with better quality, especially resistant to environmental stresses, which appears impossible with conventional approaches because it is highly time-consuming, less selective, and has limitations towards genetic transformation, species barriers, and various biological processes in wheat [9]. However, using different biotechnological techniques can play a substantial role in achieving the desired goals of wheat production [10]. Therefore, enhancing wheat production by using tissue culture protocols like callus induction and regeneration is necessary to meet the current food shortage [11].
Various explants have been established for wheat callus cultures, such as segments of a leaf [12], anthers [13], microspores, and immature [14] and mature embryos [15], which showed variable responses for callus induction and regeneration. During in vitro studies, the highest frequency of regenerated plants was reported in immature embryos and inflorescences. An immature embryo is a better explant source for regeneration that requires optimum growth facilities and time [16]. Mature embryos are available throughout the year and can be used directly or dissected [12]. The immature embryo is the most commonly used explant for wheat callus induction, while mature and well-differentiated tissue faces difficulty in re-entering the cell cycle to divide; however, an increase in metabolic activities of cells may enhance the capability of the mature embryo to regenerate easily [17].
In vitro tissue culturing induces recombinant DNA and somaclonal alterations, leading to increased crop production and higher nutritional values by callogenesis and regeneration. The upright and high percentage of callus induction depends upon an efficient sterilization process, media composition, pH, phytohormones, type of explant, and incubator conditions [18]. Various combinations of hormones are being utilized to enhance regeneration and the rate of callogenesis [19]. The levels of plant hormones in the tissue culture system are important for regulating growth and morphogenesis. The plant growth regulators frequently utilized for regeneration in plant tissue culture are cytokinin and auxin. The auxin-to-cytokinin ratio regulates the plant cell formation pathway and culture protocol [20]. Usually, higher auxin concentrations and low cytokinin levels in the media stimulate extensive cell growth and callus production. Shoot regeneration is better on the lower concentrations of 2,4-D or a hormone-free medium than on a medium with IAA (indole acetic acid) and BAP (6-benzylaminopurine). Plant cell and tissue culture offer helpful methods for maintaining and flourishing genotypes using appropriate explants that promote genetic recombination for breeding [21].
Recombination in wheat is problematic due to the unavailability of appropriate explants with higher callogenesis and regeneration rates; therefore, there is a need to optimize a culture protocol for this purpose [12]. We performed our experiment using different plant hormones on those wheat varieties on which tissue culture had not been performed. This study aimed to determine wheat varieties’ callogenesis and regeneration potential by devising an effective protocol for inducing callus in an MS medium with several plant hormones. The following questions were addressed: (a) What are the optimal conditions for the induction of callus in MS media supplemented with different plant hormones?
(b) What are the optimum levels of plant hormones for the regeneration of wheat varieties? (c) selection of wheat varieties that are best for tissue culture.
Materials and Methods
The trial was conducted at the Agricultural Biotechnology Research Institute, AARI, Faisalabad, Pakistan, from 2021 to 2022. The study area lies at latitude 31º41’ N and longitude 73º12’ E. Immature embryos of 5 high-yielding wheat varieties (Akbar-2019, Arooj-2022, Dilkash-2020, Subhani-2021, and MH-2021) were taken from AARI (Ayub Agricultural Research Institute), Faisalabad, Pakistan, for callus induction and regeneration studies. All the procedures were done under a laminar flow cabinet.
Source of Material and Treatment
Immature seeds were the source of explants and culture in MS media [22]. Three hormones, i.e., 2,4-D, IBA, and NAA, with five levels each (1 to 5 mg/L), were applied for callus induction. The callus was subjected to shoot and root regeneration using three levels of kinetin, i.e., 0.5 mg/L, 1 mg/L, and 1.5 mg/L, and two levels of NAA, i.e., 0.5 mg/L and 1 mg/L, respectively.
Surface Sterilization of the Explant
The immature seeds were sterilized with distilled water 3 times. The explant was disinfected by dipping it in 5% bleach for 30 min., shaking it well, and then sterilizing it with 90% ethanol for 1 min. Explant surface sterilization was performed with autoclaved distilled water 3-5 times until the sterilant was completely removed.
Callus Induction and Regeneration
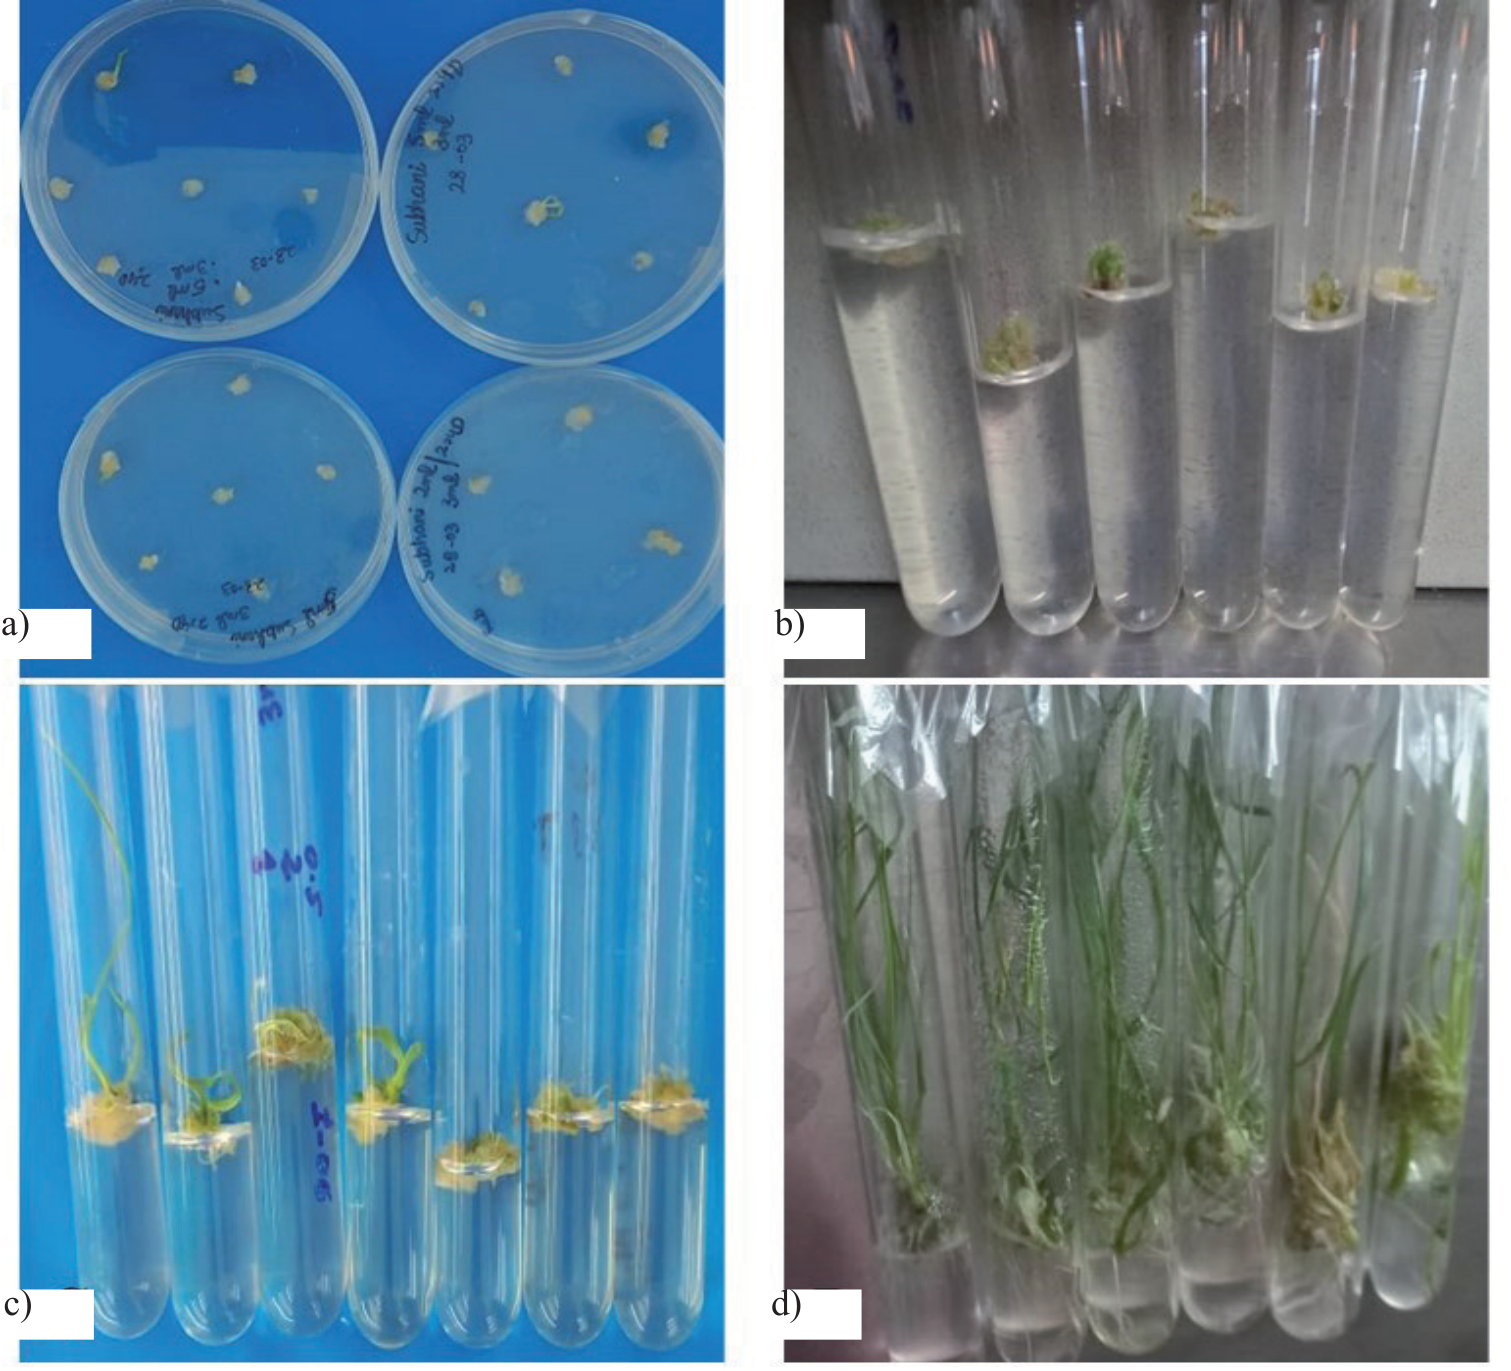
Sterilized forceps and a knife were used for the removal of the immature embryo from the seed and placed on MS + callus media having five levels of the 2,4-D hormone (1 mg/L, 2 mg/L, 3 mg/L, 4 mg/L, and 5 mg/L), phytagel 2 g/L, and 30 g/L sucrose. The medium’s pH was maintained from 5.7 to 5.8, and autoclaved for 20 min. at 15 lbs/inch2 pressure, and 121ºC temperature. Explants were cultured at a temperature of 20±1 to 27±1ºC throughout periods of light and darkness, and the callus induction percentage from the cultured embryo was noted. Calli were shifted to freshly prepared MS media with the same hormone to maintain callus and further propagation. Callus media was refreshed after 14 days. A similar procedure was carried out for callus induction in NAA and IBA hormones, but callus induction was not seen at any level of IBA or NAA. After callus induction in 2,4-D media, the callus was shifted to regeneration media having various concentrations of kinetin and NAA along with 30 g sucrose and 2 g/L phytagel (Fig. 1). The traits recorded for callus were callus induction and its fresh and dry weights; however, shoot and root regeneration traits were shoot length, root length, root percentage, number of shoots per plant, and their fresh and dry weights. Weights were recorded using a digital balance, and lengths were measured with the help of a measuring tape.
Statistical Analysis
All the determinations were made in three replicates from the completely randomized design (CRD). Software Statistix 8.1 assessed the significant differences among the wheat varieties at varying kinetin, NAA, and 2,4-D concentrations. MS EXCEL was used to present the data. PCA was performed to determine the correlation among wheat varieties with callus formation and root and shoot regeneration. The graphical presentation was done using ggplot2, factoextra, and factominer packages in R software (4.0.2).
Results and Discussion
Callus Formation
Different concentrations of three hormones, i.e., NAA, 2,4-D, and IBA, were added to MS media separately for callus initiation; however, callus initiation was observed by the 2,4-D hormone only after nearly 14 days, which shows that 2,4-D is an effective hormone for callus development [23]. The induction of callus was observed through visual inspection and was characterized by the appearance of an undifferentiated mass of cells. All the callus traits showed highly significant (p≤0.001) variation among wheat varieties, 2,4-D, and the interaction between varieties and 2,4-D (Table 1).
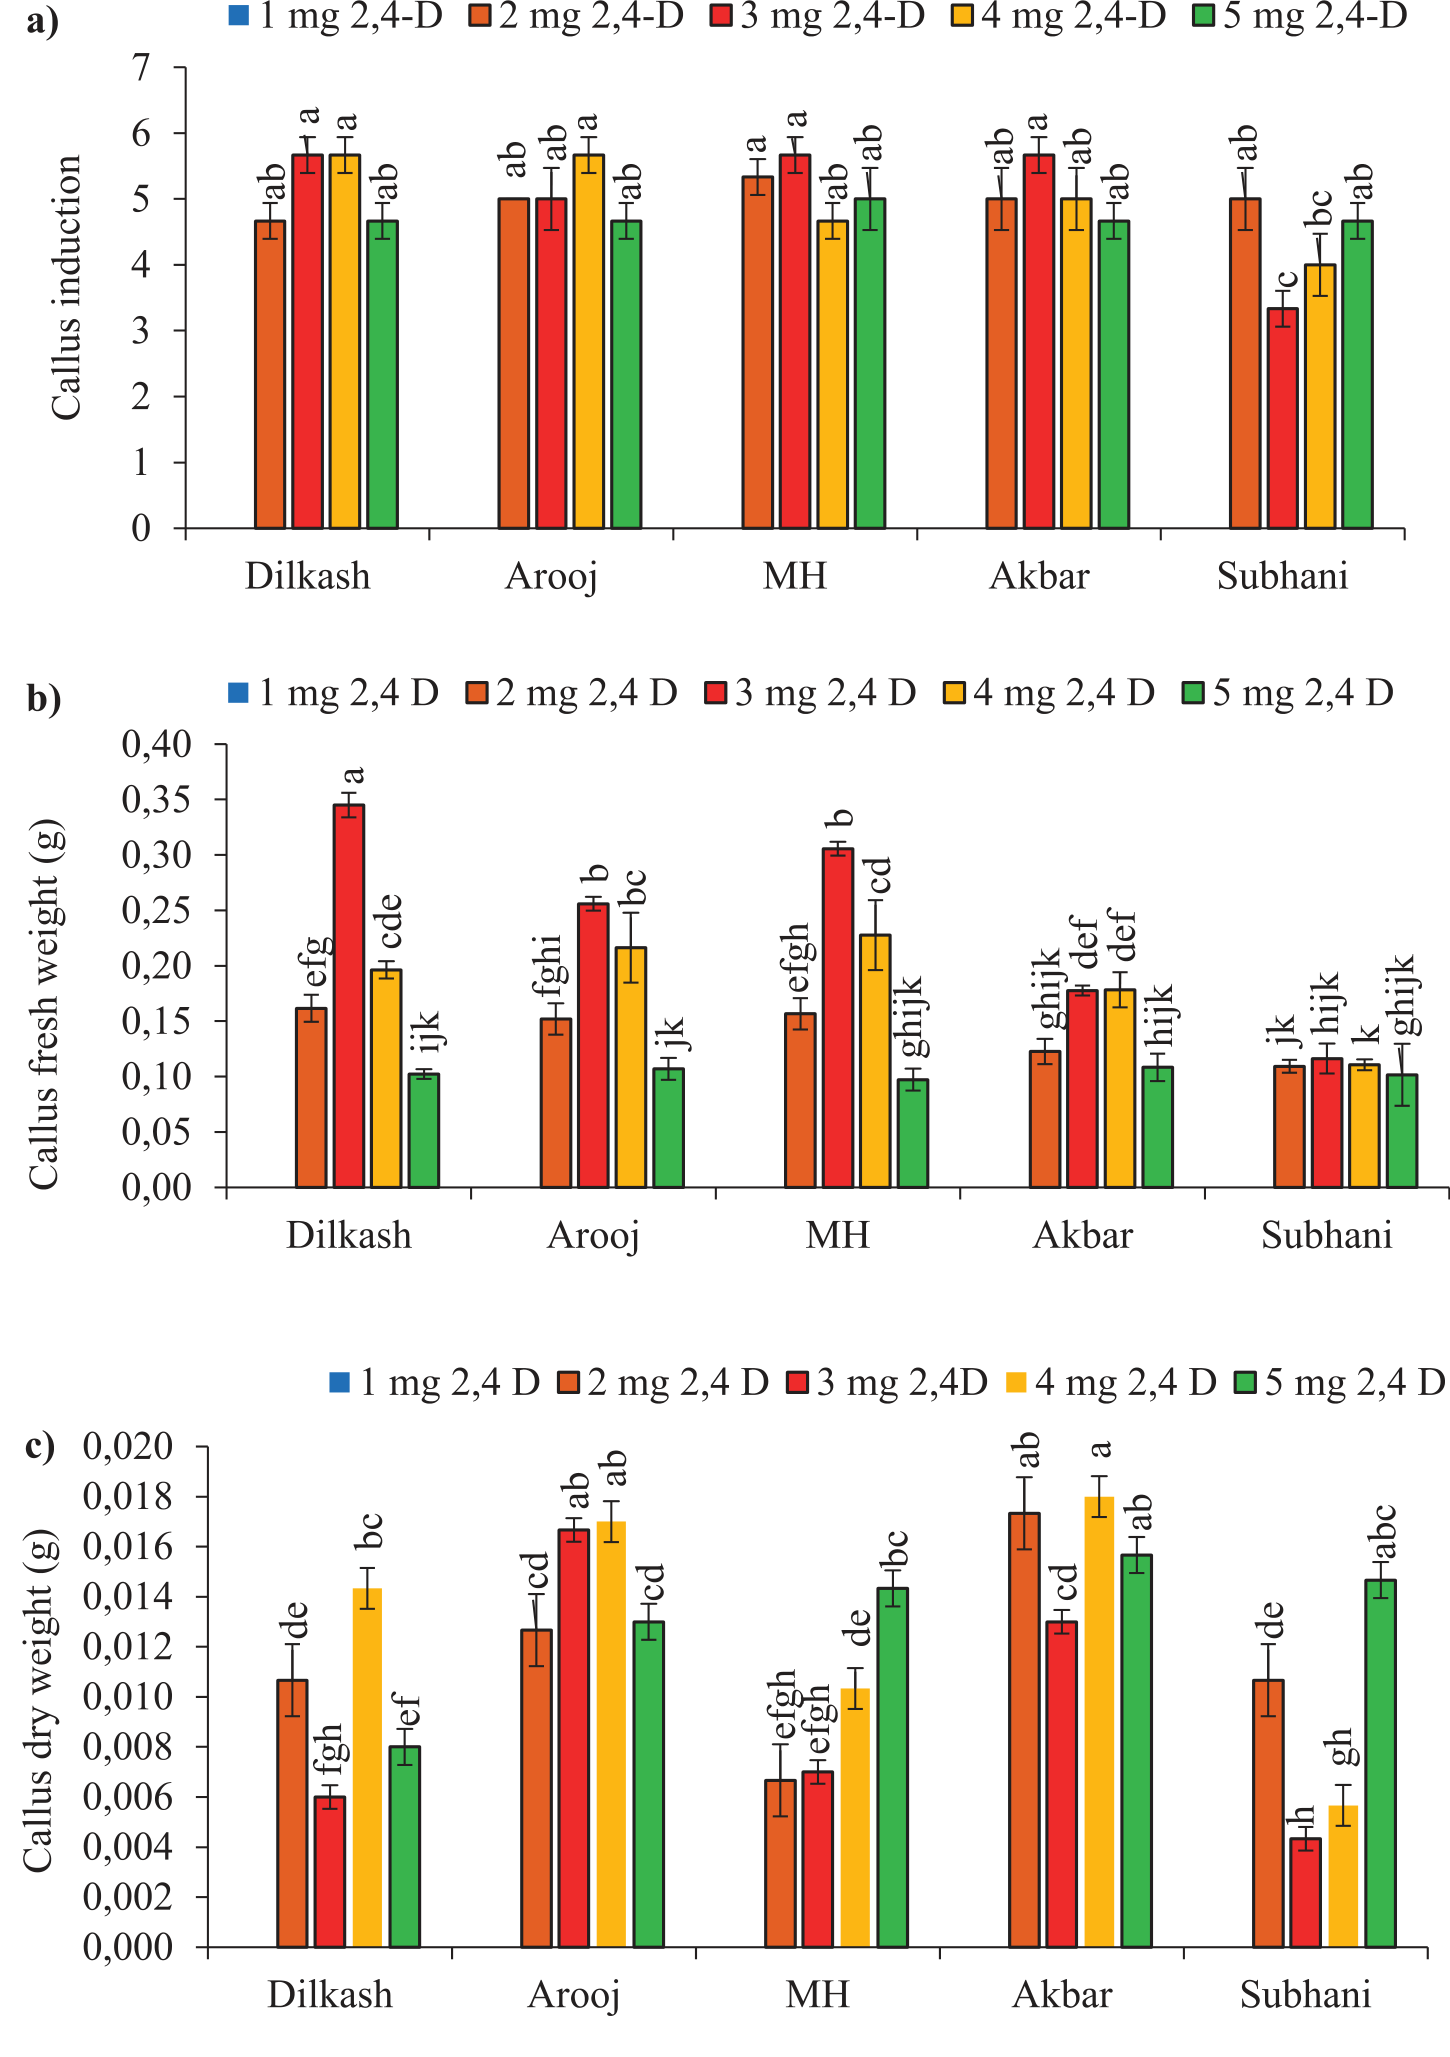
All the wheat varieties responded differently to 2,4-D concentrations in the media. Callus formation wasn’t recorded in all wheat varieties at the lowest concentration of 2,4-D, i.e., 1 mg/L. At 2 mg/L of 2,4-D, callus induction was highest in MH, followed by Arooj, Akbar, Subhani, and Dilkash varieties. The highest callus formation was recorded at 3 mg/L 2,4-D in Dilkash, MH, and Akbar. Arooj and Dilkash varieties showed the maximum callogenesis at 4 mg/L (Fig. 2a). Nawaz et al. [24] reported that callus development was negligible at 1 mg/L 2,4-D, and lower callus induction was noted at 5 mg/L. Our findings also coincide with the results of Patel et al. [25] and Mahmood et al. [26] in wheat; they recorded that 3 mg/L of 2,4-D was the best, and as the amount of 2,4-D increased, the callus initiation rate gradually decreased. The outcomes of the current study specified that the induction of callus depends not only on the different treatments of 2,4-D but also on the varietal differences present in wheat varieties, and our results are consistent with the earlier findings of [27] and [28]. The varietal differences normally result from variations in internal hormonal levels and genetic makeup [29].
Fig. 1.
Some representative pictures of wheat varieties showing a) callus formation and (b-d) root and shoot regeneration.
An increase in callus fresh weight was noted by boosting the level of 2,4-D up to 3 mg/L. In Dilkash at 3 mg/L of 2,4-D, callus fresh weight was highest, followed by MH and Arooj. The highest values of fresh weights were recorded in MH, Arooj, and Dilkash at 4 mg/L of 2,4-D. The lowest fresh weights were noted in the Subhani variety at every level of 2,4-D. In general, the results demonstrated that raising the concentrations of 2,4-D positively affected the fresh weight up to 3 mg/L. After that, at higher levels (4 and 5 mg/L), fresh weights were reduced (Fig. 2b). Maximum callus dry weight was noted at 2 mg/L of 2,4-D in Akbar, followed by Arooj, Subhani, and Dilkash, while minimum callus dry weight was recorded in MH. At 4 mg/L, the dry weight of the callus was the highest in Akbar, followed by Arooj and Dilkash, and the lowest value was recorded in Subhani. The highest callus dry weight was observed in Arooj, and the lowest dry weight was noticed in Subhani at 3 mg/L of 2,4-D (Fig. 2c). Callus is used in various biotechnological aspects; therefore, the wheat varieties having higher values of callus fresh and dry weights possess a greater ability to grow [30]. Yadav et al. [31] showed that 2,4-D was the most potent for in vitro callogenesis in wheat among other auxins. Similarly, Kumar et al. [32] reported that 2,4-D was superior to NAA or IBA for callus formation. One of the most potent synthetic auxins, 2,4-D, is essential to several in vitro techniques, including callogenesis, embryogenesis, organogenesis, and shoot regeneration [33].
Table 1.
Analysis of variance (F-ratios) for callus traits of wheat treated with 2,4-D.
Fig. 2.
Effect of different concentrations of 2,4-D hormone on a) callus induction, b) callus fresh weight, and c) callus dry weight of 5 wheat varieties (Dilkash, Arooj, MH, Akbar, and Subhani). Values represent means ± S.E. Significant differences were measured by the least significant difference (LSD) and indicated by different lowercase letters. S.E. stands for standard error.
Role of Kinetin in Shoot Regeneration
Cytokines best promote plant cell division and cell differentiation, as they perform a major role in plant tissue culture [34]. It promotes the growth of shoots from the meristematic tissues and encourages the development of multiple shoots [35]. Kinetin, a synthetic cytokinin, was used to stimulate shoot formation. This protocol was devised to check the level of kinetin, which provides maximum results in shoot induction. All shoot regeneration traits showed highly significant (p≤0.001) results for varieties and kinetin. The interaction between varieties and kinetin represented highly significant variations (p≤0.001) for shoot length and number of shoots per plant, while significant (p≤0.05) results were obtained for fresh and dry weights (Table 2).
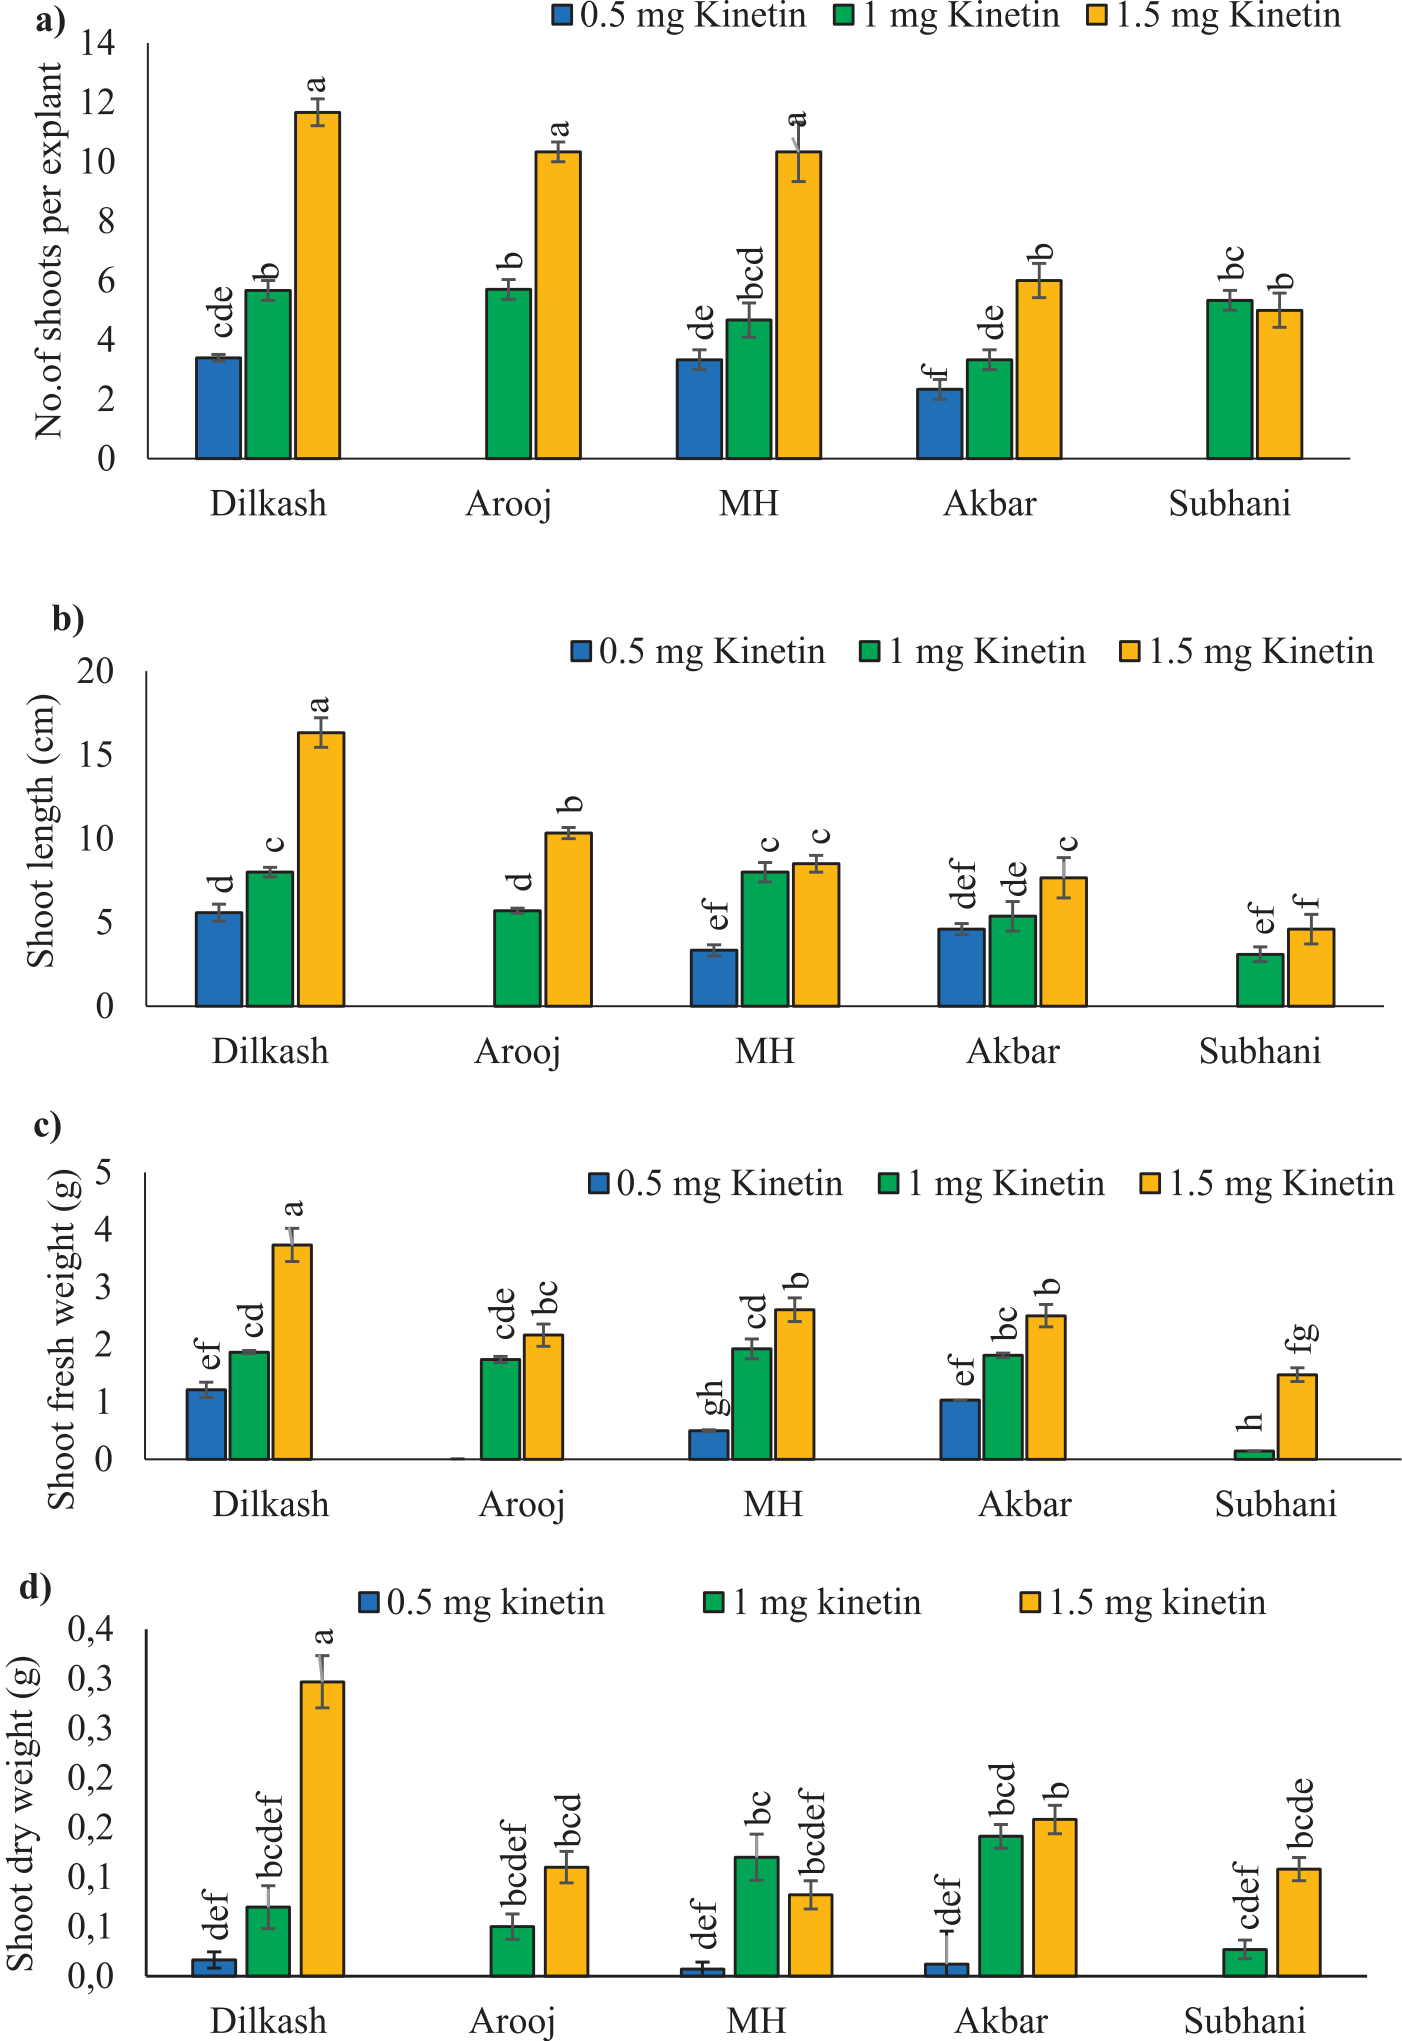
It was noted in all varieties that by boosting the concentration of kinetin up to 1.5 mg/L, the number of shoots formed was improved. However, Dilkash, Arooj, and MH varieties showed more formation of shoots as compared to Akbar and Subhani (Fig. 3a). Our study is contradictory to the findings of Mahmood et al. [26], who tested the greatest regeneration ability of wheat varieties at 1 mg/L kinetin and after that at 1.5 mg/L kinetin. In comparison, El Sayed et al. [36] studied the MS medium provided along with 0.5 mg/L kinetin and 0.5 mg/L BAP, which led to maximum regeneration. Rahman et al. [37] revealed that maximum regeneration in wheat was achieved at 1 mg/L kinetin. Conflicts may result from diverse explant sources, genetic material under research, external factors, and variability in cultural conditions [26, 38]. The environment can influence the callus’s ability to regenerate by changing the internal hormonal balance of the explant [38].
Shoot length and fresh weight of shoots were maximum at 1.5 mg/L in all varieties compared to the lower levels, i.e., 0.5 and 1 mg/L kinetin. Dilkash exhibited better performance in terms of shoot length and fresh weights; however, Subhani showed a poor response (Fig. 3b) and c)). The highest shoot dry weight was noted at 1.5 mg/L in Dilkash, followed by Akbar. The lowest dry weights were noted at 0.5 mg/L kinetin (Fig. 3d). Plants with better growth features show better survival potential in both normal and stressed environmental conditions [39].
Root Formation from Shoots by Different Levels of NAA
Auxins are the primary plant growth regulators that promote root growth in many plant species. The role of NAA, a synthetic auxin, in root induction at different levels was observed. All the root traits showed highly significant variations (p≤0.001) among wheat varieties and NAA levels, except root percentage, while the interaction between NAA and varieties represented highly significant variations (p≤0.001) for root fresh and dry weights (Table 3).
Maximum root formation was noted at 1 mg/L NAA (Fig. 4a). Moreover, according to Pathak et al. [40], NAA at 1 mg/L provided the best rooting response. Maximum root length was recorded in Dilkash at both levels of NAA; however, minimum root length was observed in Arooj at both levels of NAA (Fig. 4b). The highest root fresh weight was recorded in Dilkash at 1 mg/L NAA, while in Arooj and MH intermediate root fresh weight was noted, whereas Subhani and Akbar showed the lowest root fresh weight at 1 mg/L (Fig. 4c). The highest root dry weight was recorded in Dilkash and MH at both levels, i.e., 0.5 mg/L and 1 mg/L NAA, while the root dry weight was the lowest in Subhani at these levels (Fig. 4d). NAA is the most effective plant growth hormone for inducing root formation in several plants [37, 41]. Multiple investigations have shown that lower NAA levels of 0.5-3 mg/L are required for attaining optimum rooting [24, 42]. Waseem et al. [43] reported that the lowest concentration of NAA (0.5 mg L-1) produced the greatest number of shoots per explant, leaves, and nodes per shoot when applied alone, suggesting its superiority over all other concentrations of NAA. It was also noted in Chrysanthemum that a higher NAA concentration in MS media lowered the rate of multiplication [44]. NAA treatment boosted root production in azalea cultivars, but the roots were short and fragile because high concentrations of NAA may hinder root elongation [45].
Principal Component Analysis (PCA)
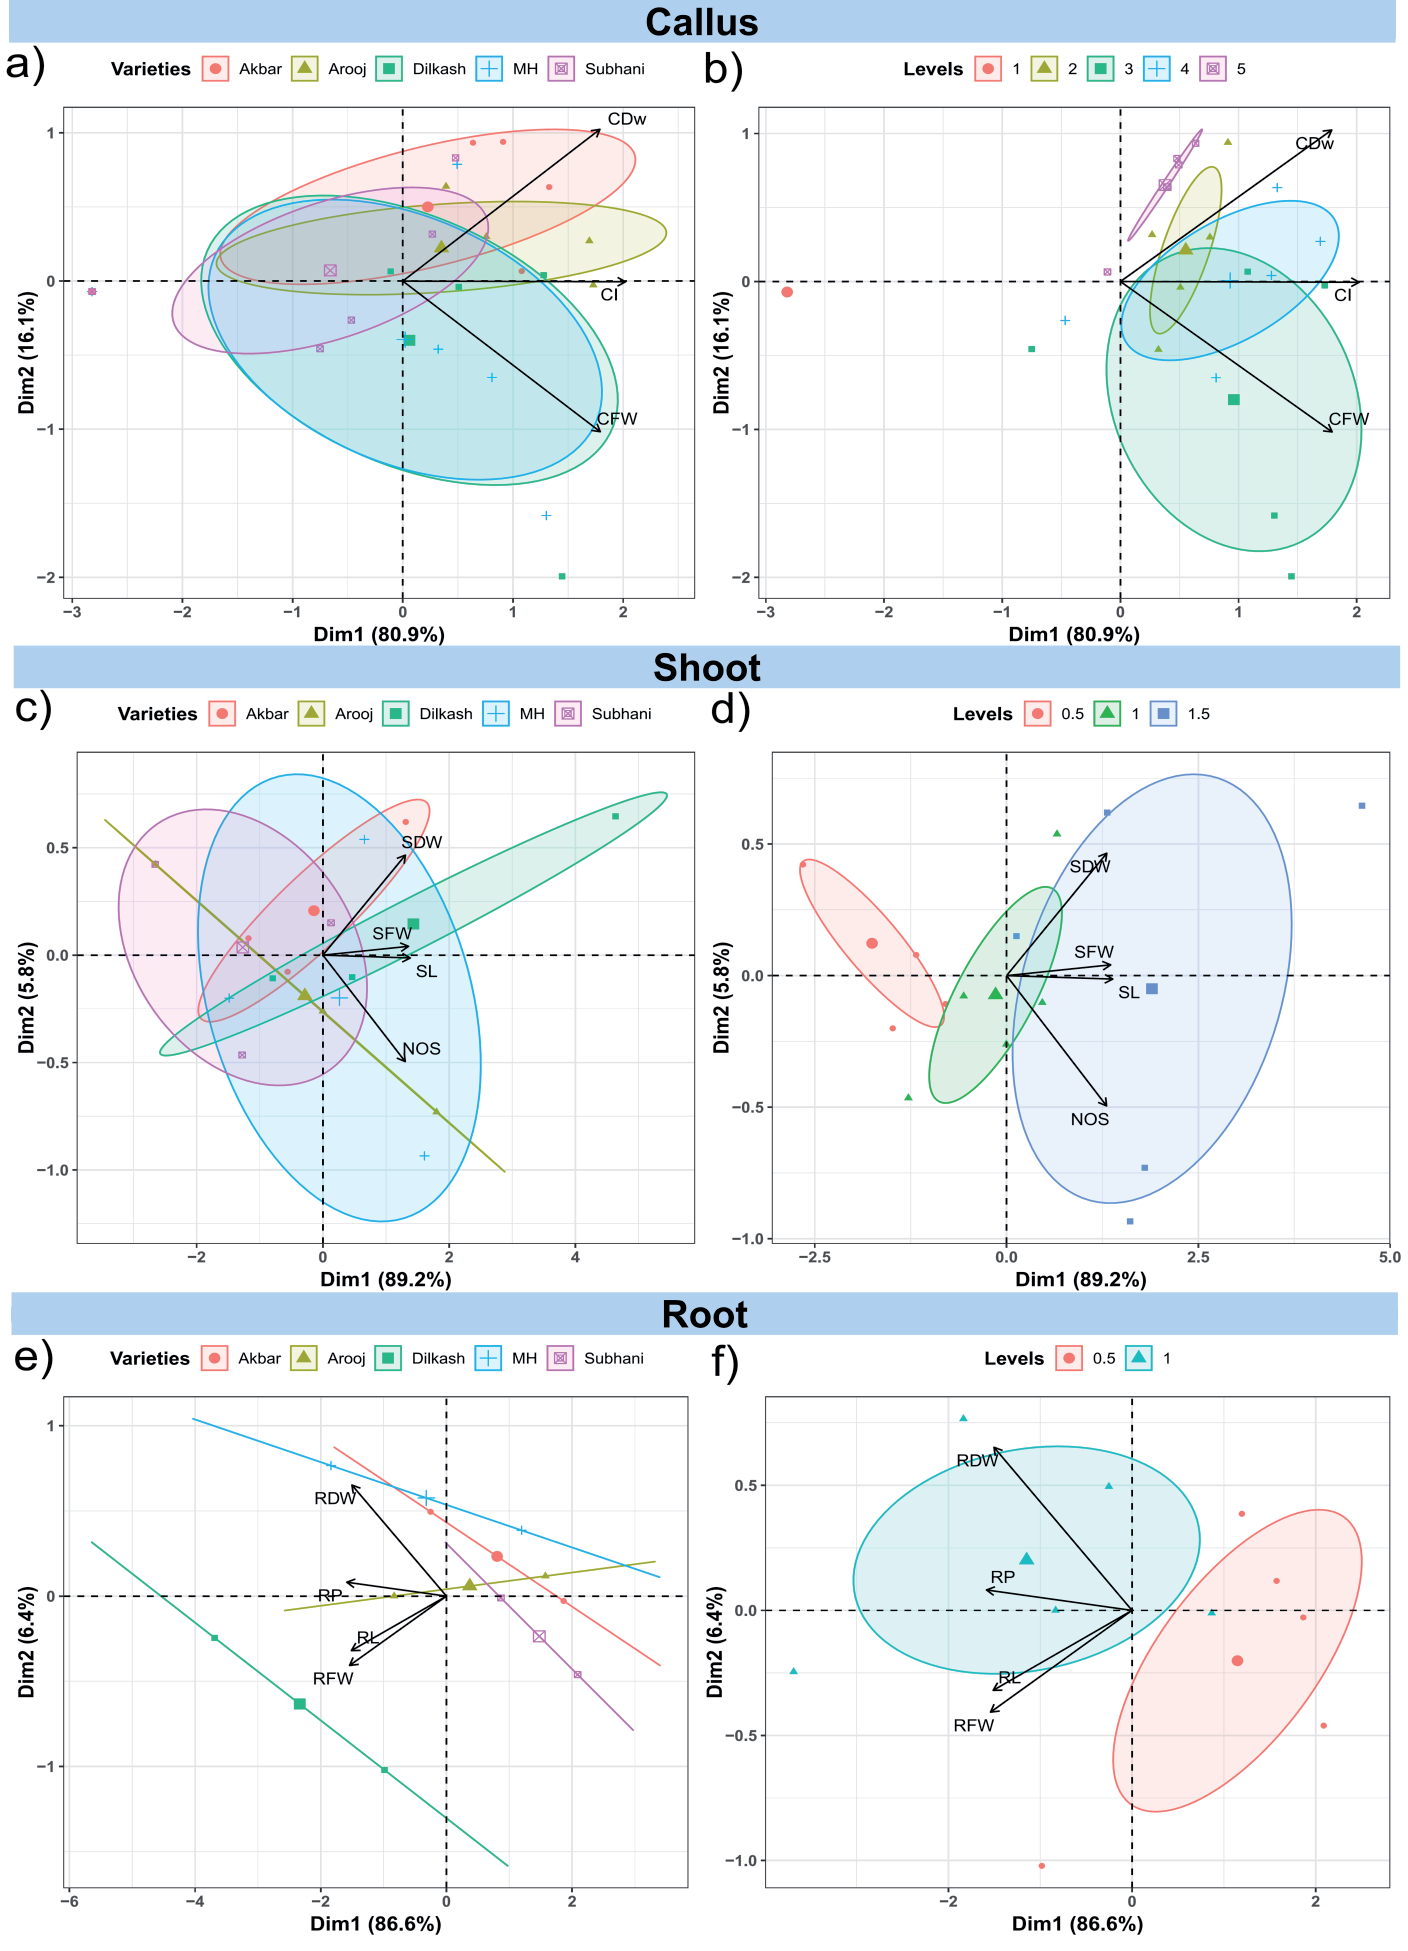
The PCA demonstrated a significant impact of the 2,4-D hormone in wheat varieties for callus parameters (Fig. 5a) and b)). The PCA components, i.e., Dim1 and Dim2, exhibited a 97% total variation. Dim1 contributed 80.9% and Dim2 16.1% of the variation. Akbar reflected the highest value of CDW and the lowest CFW. Subhani showed lower values for all parameters than the others. Most of the influence of CFW was observed in Dilkash and Arooj (Fig. 5a). CFW was significantly influenced at a 3 mg/L concentration with positive eigenvalues; however, for CI, all levels of 2,4-D contributed equally except 5 mg/L 2,4-D (Fig. 5b)). Dim1 explained 80.9% of the total obtained variation; the first dimension defined CFW, CDW, and CI, so Dim1 alone should be a good indicator of the effect of the 2,4-D hormone.
Table 2.
Analysis of variance (F-ratios) for shoot regeneration traits of wheat treated with kinetin.
Fig. 3.
Effect of different concentrations of the kinetin hormone on a) number of shoots per explant, b) shoot length, c) shoot fresh weight, and d) shoot dry weight of 5 wheat varieties (Dilkash, Arooj, MH, Akbar, and Subhani). Values represent means ± S.E. Significant differences were measured by the least significant difference (LSD) and indicated by different lowercase letters. S.E. stands for standard error.
Shoot regeneration PCA demonstrated the role of different levels of kinetin on wheat varieties in which Dim1 and Dim2 exhibited 89.2% and 5.8% variations, respectively (Fig. 5c) and d)). Akbar and Subhani showed different results regarding SDW and NOS, as Akbar has relatively higher SFW, SDW, and SL values, while Subhani possesses lower values for all parameters (Fig. 5c). The lowest scores for all parameters were shown at 0.5 mg/L kinetin. 1.5 mg/L kinetin showed a higher value on SFW, SDW, NOS, and SL. The strongest positive correlation exists between SFW and SL; however, a negative correlation was noticed between SDW and NOS (Fig. 5d).
Root regeneration PCA demonstrated the influence of different concentrations of NAA hormone on wheat varieties, in which Dim1 and Dim2 contributed 86.6% and 6.4% variations (Fig. 5e) and f)). A 1 mg/L concentration of NAA exhibited higher values of RDW with positive eigenvalues and RFW and RL with negative eigenvalues. However, no major contributor was found under 0.5 mg/L NAA treatment. A strong positive correlation exists between RL and RFW, and a negative correlation was noted between RDW and RFW.
Table 3.
Analysis of variance (F-ratios) for root regeneration traits of wheat treated with NAA.
Fig. 4.
Effect of different concentrations of NAA hormone on a) root percentage, b) root length, c) root fresh weight, and d) root dry weight of 5 wheat varieties (Dilkash, Arooj, MH, Akbar, and Subhani). Values represent means ± S.E. Significant differences were measured by the least significant difference (LSD) and indicated by different lowercase letters. S.E. stands for standard error.
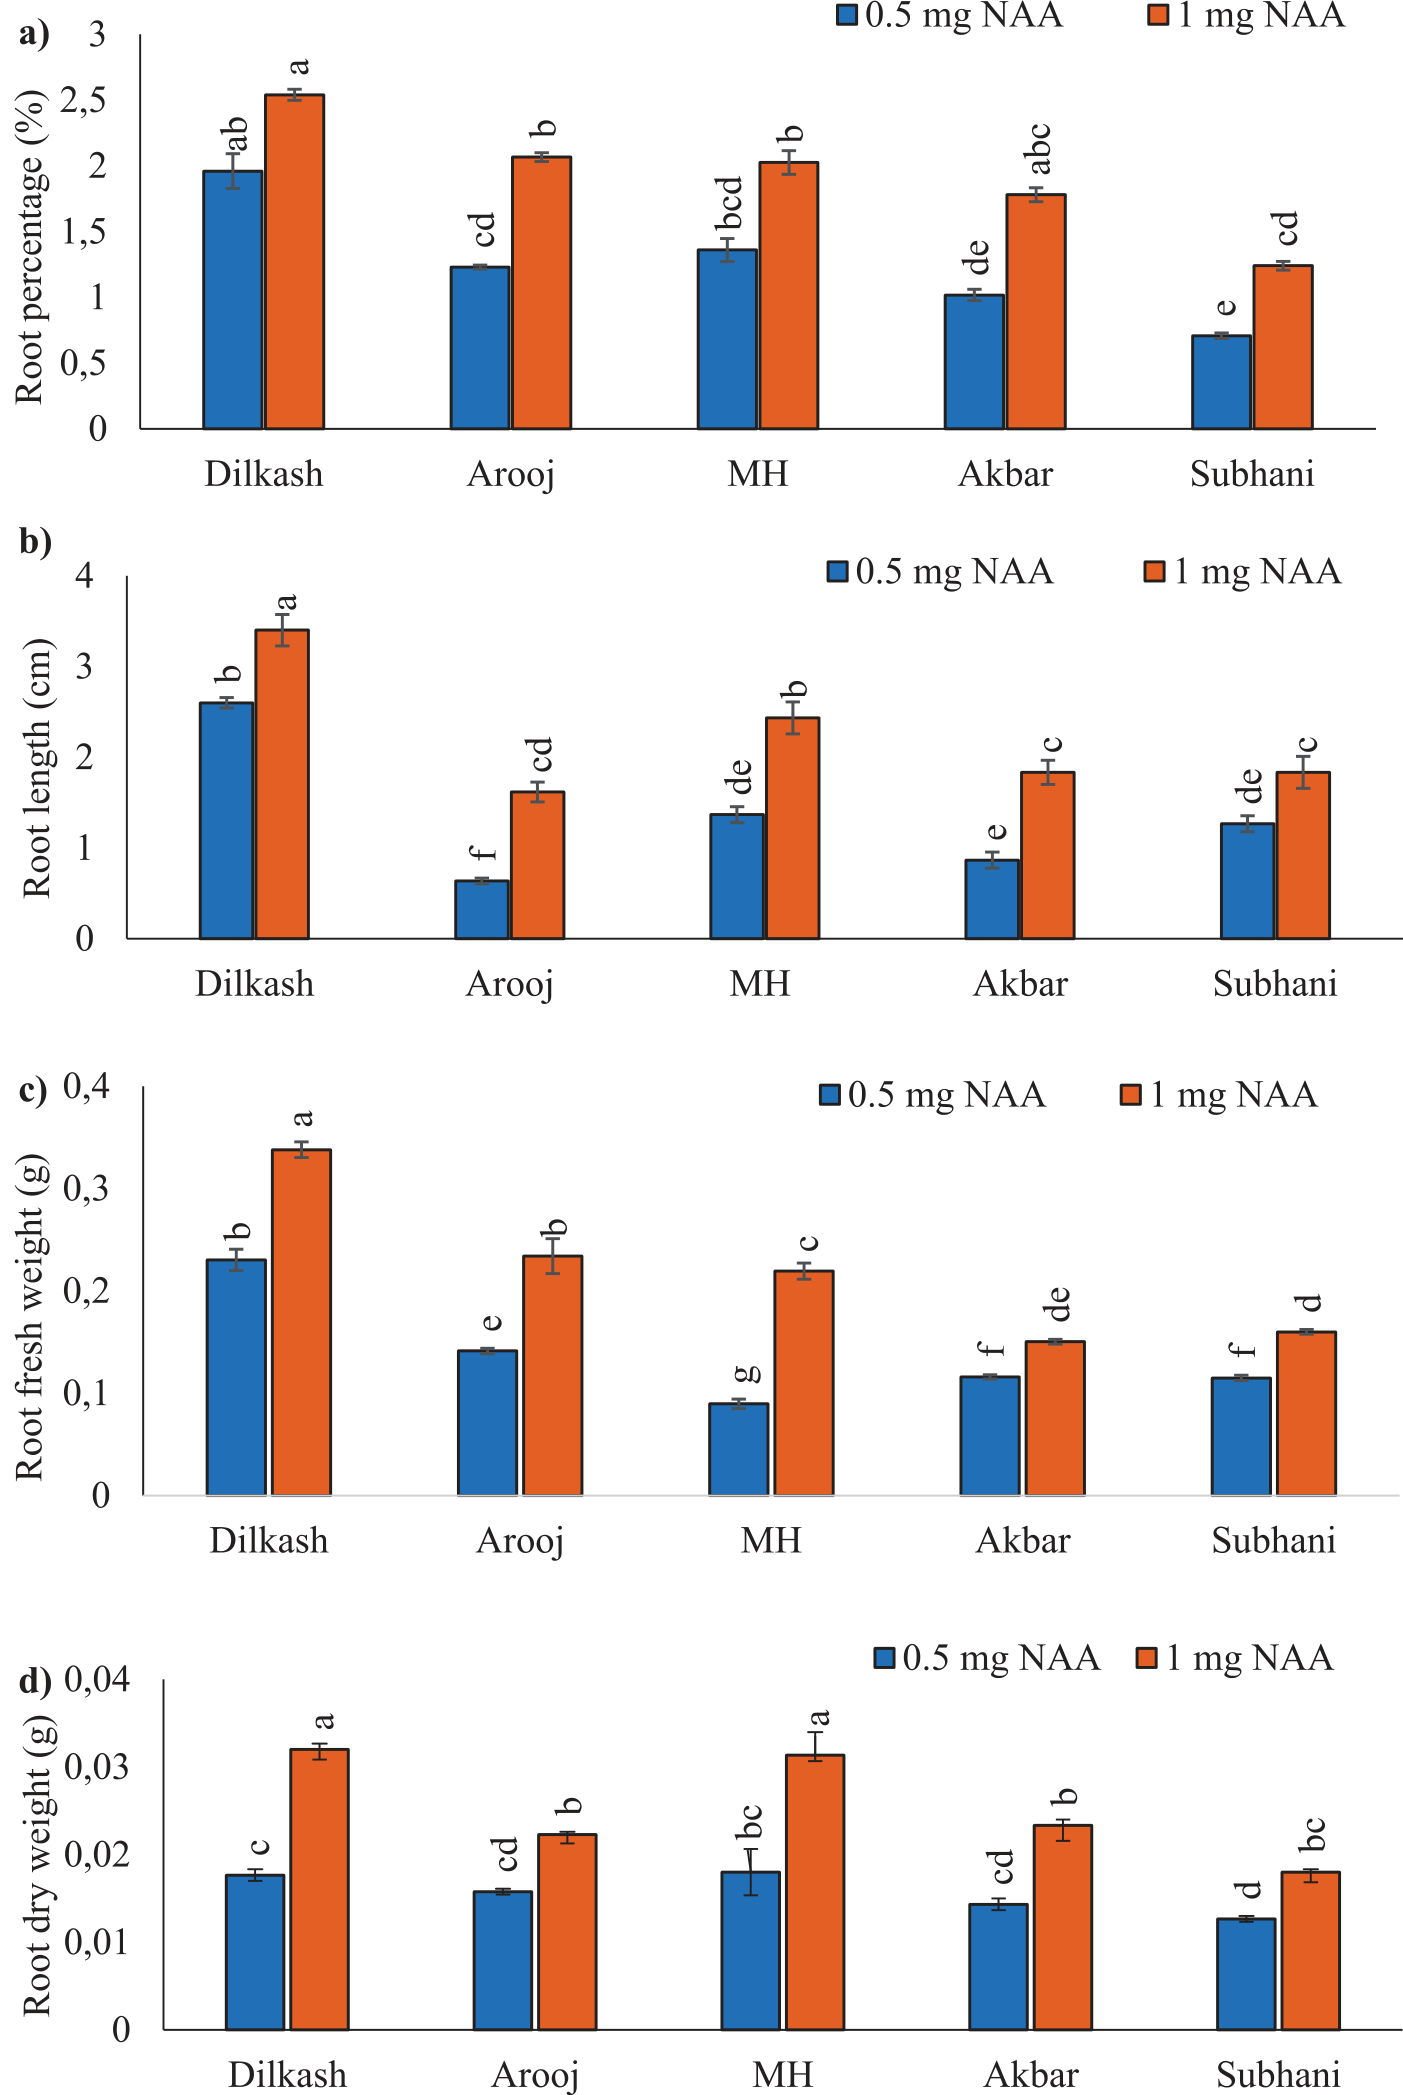
Fig. 5.
Principal Component Analysis (PCA) of 5 wheat varieties for callus formation and root and shoot regeneration; a) and b): PCA represents the effect of 2,4-D treatment on 5 wheat varieties for callus induction (CI), callus fresh weight (CFW), and callus dry weight (CDW); c) and d): PCA plot of five wheat varieties represent the effect of kinetin on shoot regeneration parameters, i.e., shoot dry weight (SDW), shoot fresh weight (SFW), shoot length (SL), and number of shoots (NOS); e) and f): PCA plot represent NAA effect on root regeneration parameters, i.e., root dry weight (RDW), root fresh weight (RFW), root length (RL), and root percentage (RP).
Conclusions
The study concluded that using immature embryos as explants results in a higher rate of callus initiation and that plant regeneration is feasible in wheat. All wheat varieties behaved differently for callus induction and regeneration. The difference in responses was due to the different levels of phytohormones and the different genetic makeup of wheat varieties. Hormones like NAA and IBA do not influence the development of the callus. It was concluded that 3 mg/L 2,4-D is best for the induction of callus, 1.5 mg/L kinetin for shoot regeneration, and 1 mg/L NAA for root regeneration in all wheat varieties except Subhani and Akbar.

