

Introduction
Boron (B) is an essential micronutrient for the normal growth and development of plants, which is required for the proper maintenance of the physiological and biochemical processes of the plants. Their deficiency or excess affects these physiological and biochemical processes and is hence responsible for the decline in plant growth and productivity [1]. The primary function of boron is cell wall synthesis, along with the maintenance of its structure and integrity. An optimum quantity of boron is required at all stages of plant growth, from the vegetative to the reproductive stage, for enhancing flower production and retention, followed by the germination of pollen along with pollen tube elongation, and finally fruit and seed development [2]. Optimum use of boron fertilizer is necessary to obtain high yields and quality fruit crops. Deficient and toxic levels of boron are associated with plant disorders and a reduction in the yield of crops. To encounter sufficiency, deficiency, and toxicity levels of boron in crop plants based on a definite critical value is a major challenge because sufficiency and toxicity are narrower compared to other nutrient elements [3].
Boron deficiency affects the synthesis of proteins by regulating hormone metabolism, viz., auxin, calcium translocation, and the production of growth regulators, all of which are also crucial for membrane metabolism and function [4]. B deficiency in plants restricts root elongation, along with flower deformation and fruit formation, because of inhibition of cell division in the meristematic region, while adequate B supply promotes healthy root development. Reduced tree vigor and growth are due to a boron deficit, while a severe deficiency may cause twig die-back, leaf rosettes formation, and bud drop. During the reproductive stage, empty pollen grains and poor pollen vitality with a reduced number of flowers per plant are some of the common deficiency symptoms of boron [5]. The primary effect of B deficiency seems to be disruption of the normal functioning of the apical meristem, with changes in auxin metabolism, lignification, phenol accumulation, and sucrose transport being secondary effects, while its excessive accumulation may cause B phytotoxicity [6]. Janaki et al. (2020) reported boron deficiency is more extensive among all plant micronutrients after zinc, which is due to a lack of boron application in nutrient management.
Esringü et al. (2022) defined that there is a narrow range between deficiency and toxicity of boron and hence possess difficulty maintaining optimum boron levels in the soil. Boron has very high potency, which means a very small quantity can cause damage like seed germination inhibition, root growth restriction, and shoot chlorosis, due to which boron is considered a hazardous element. There is one more fact about boron: monocots uptake less boron than dicots, which explains the lower boron absorption capacity of monocot roots compared to dicot roots [7]. Boron toxicity causes leaf injuries, defoliation, and shoot abnormalities. One of the distinctive symptoms of its toxicity is leaf chlorosis, i.e., loss of green color with leaf yellowing along the midrib and lateral veins. The toxicity of boron also influences different physiological processes, including cell division and elongation inhibition, cell wall disruption, and metabolic disturbance, observed that some fruits like apricots and prunes do not show any visible symptoms of boron toxicity [8].
T. aestivum L., commonly known as common wheat or bread wheat, is a widely cultivated cereal crop that belongs to the Poaceae family. It is one of the most important staple foods globally, providing a significant portion of the world’s dietary energy and protein [9]. The influence of boron on the biochemical properties of T. aestivum has gathered increasing attention in agricultural research due to its direct impact on crop yield and quality. While boron is indispensable for plant growth, both deficiency and excess can lead to detrimental effects on the physiological and biochemical aspects of plants. The intricate balance of boron in Triticum aestivum L. is crucial for optimizing agricultural practices and ensuring sustainable food production [10]. This research aims to explore the dual aspects of boron’s influence on wheat, exploring the consequences of both deficiency and toxicity on the biochemical properties of T. aestivum L.
Materials and Methods
Collection of Triticum aestivum L. Seeds
Seeds of T. aestivum L. were obtained from a reputable seed bank or supplier. A uniform seed lot was selected to ensure consistency in the experiments. The experiment was conducted in the botanical garden of Bacha Khan University, Charsadda, during the wheat growing season of 2021 [11].
Germination and Growth Conditions
The seeds were surface-sterilized using a dilute bleach solution (1% sodium hypochlorite) for 5 minutes and then thoroughly rinsed with distilled water [12].
Experimental Design:
The experiment was carried out in the field using Randomized Complete Block Design (RCBD) during the month of November under natural light conditions when the average temperature was 22ºC [13].
Germination of Triticum aestivum L. Seeds in Plastic Pots
The seeds of T. aestivum L. were sown at 2 cm depth in pots with a height of 30 cm and a 25 cm diameter. The pots were filled with (3 kg) of clay loamy soil. The soils were analyzed as having sand 27.15%, silt 19.86%, clay 52.98%, pH 6.9, water holding capacity 50.37%, bulk density 0.96 g/cc, specific gravity 4.03, and organic carbon 0.82%. No additional supplement was added to the experimental soil [14].
Experimental Setup and Treatment Levels
Control group: Plants grown in a nutrient solution without any boron supplementation are considered the control (B0).
Boron toxicity group: The pots were treated with boron applied as boric acid at the doses of B10, 20, 30, 50, and 60mg/kg.
Boron deficiency group: Plants grown in a nutrient solution with a low boron concentration. Each treatment was replicated three times in a design.
Sampling: After the treatment period (usually 15-30 days), plant samples were collected from each treatment group. Roots, shoots, and leaves were separated for analysis [15].
Biochemical analysis: The technique developed by Arnon (1949) was used to quantify the chlorophyll content of leaves. Using BSA as the standard, the protein content of leaves was determined using the Lowery et al. (1951) technique. The Bates et al. (1973) technique was used to determine the proline content of leaves. Fresh leaf sugar estimation was performed using Dubois et al.’s (1956) methodology. The technique developed by Aery et al. (2010) was used to determine the carotenoid content of leaves. The Folin-Ciocalteau technique, as described by Mahedevan and Sridhar in 1982, was used to quantify the amount of phenol in the sample. Using glycine as a reference, the technique of Sparkman et al. (1958) was used to determine the amino acid content.
Statistical Analysis
The Randomized Complete Block Design (RCBD) was used to determine all of the data that was obtained. Using STATISTIX 8.1, an analysis of variance (ANOVA) was performed on replicated data. At P 0.05, least significant differences (LSD) were used to separate means when the ANOVA revealed a statistical effect.
Results
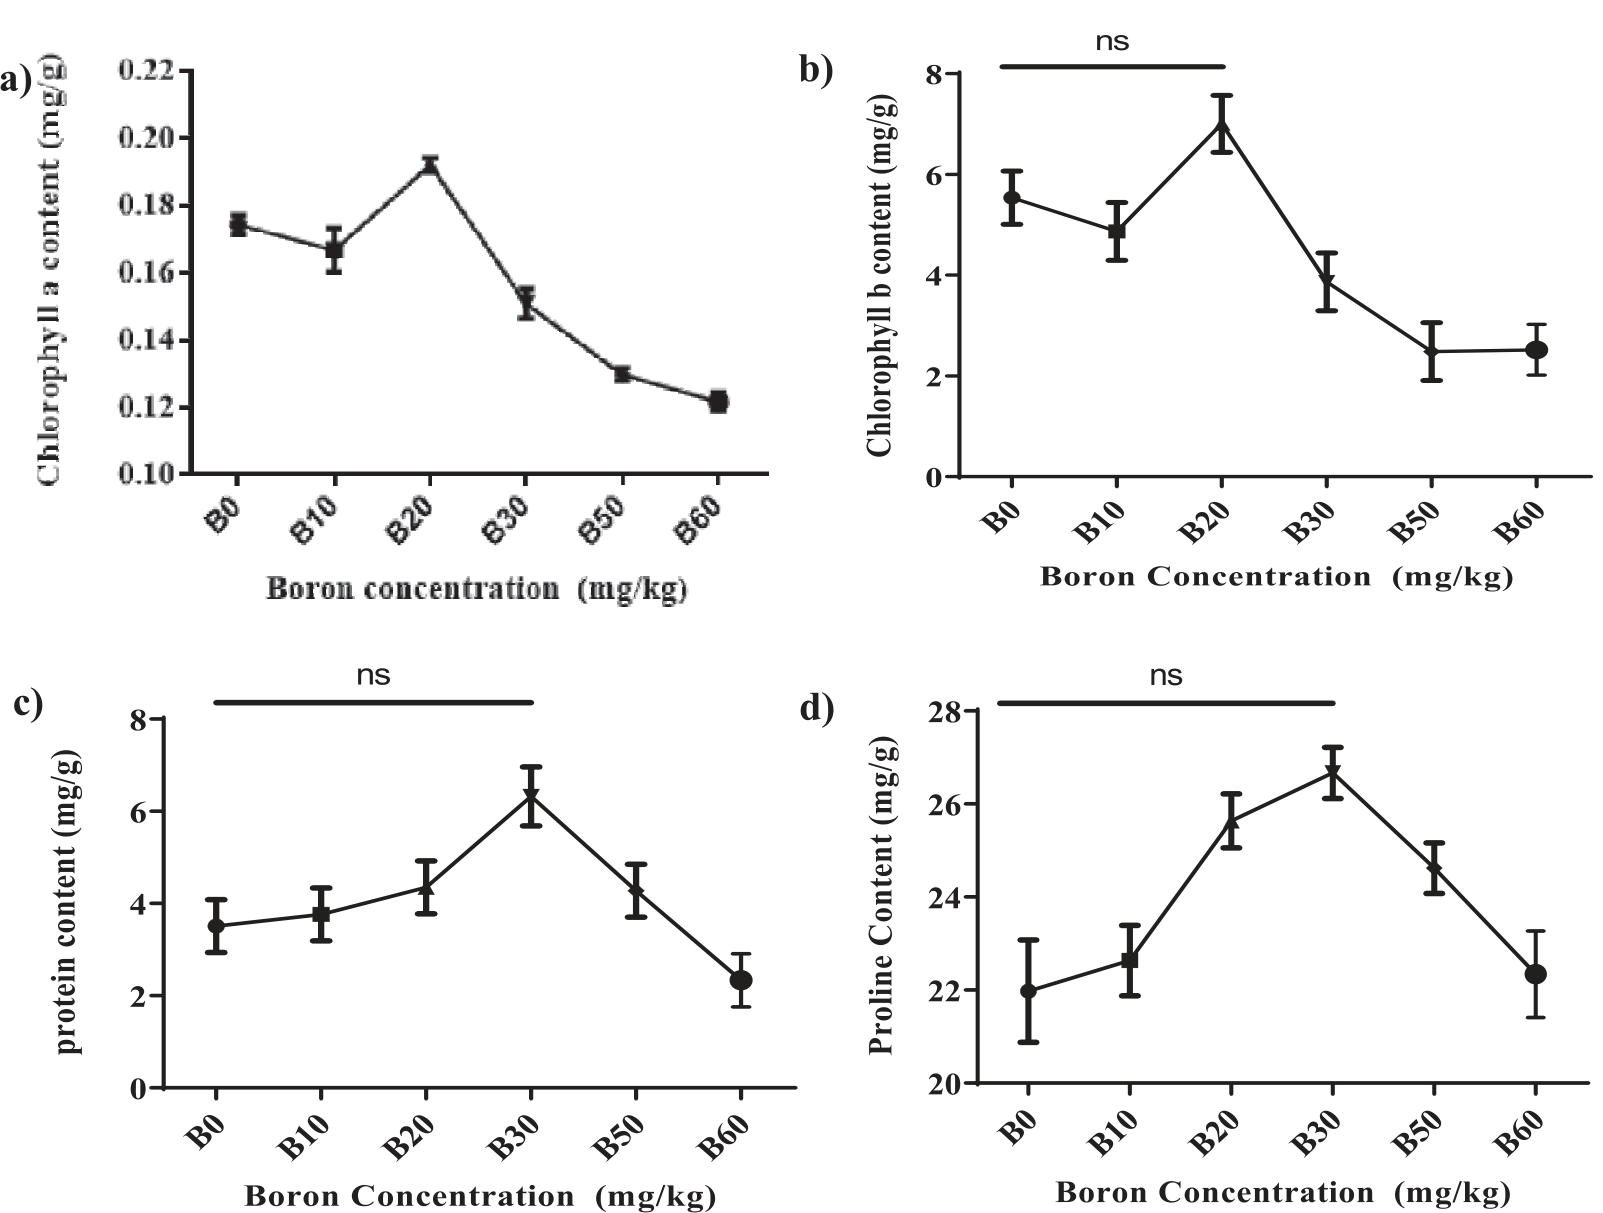
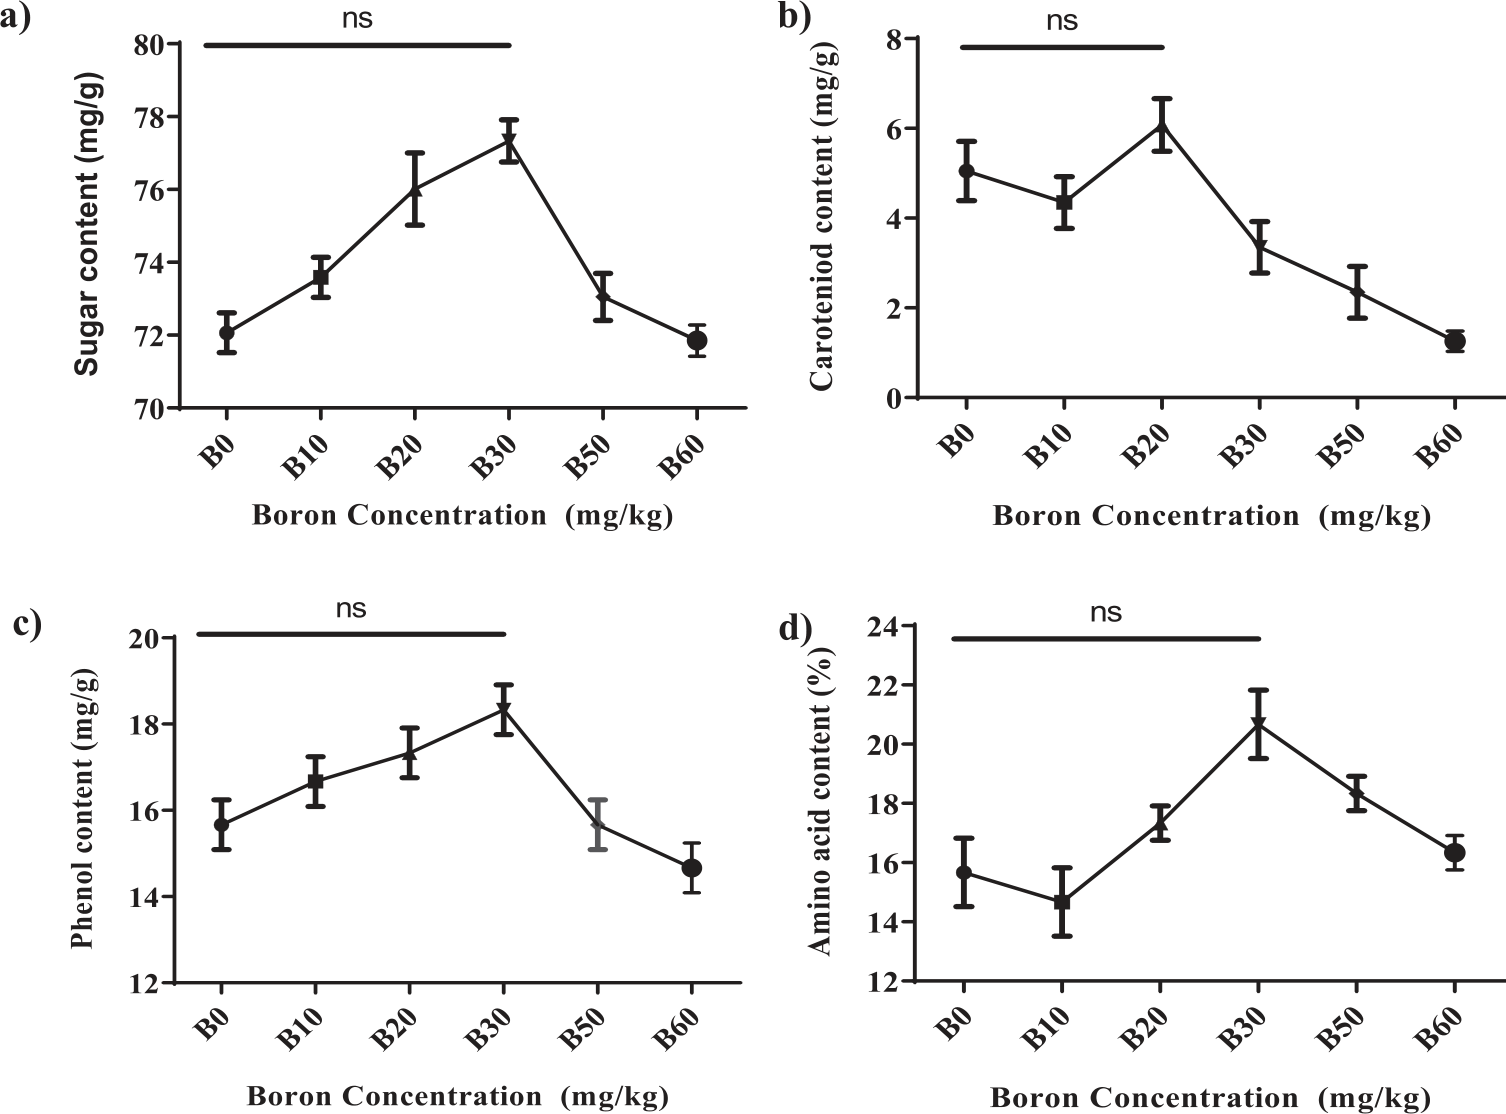
The impact of boron application on plant biochemical parameters of wheat was different; sufficient application of boron (B10, B20, and B30 mg/kg) showed a promotion in parameters, while boron deficient (B0) and boron excess (B50 and B60) showed a reduction in biochemical parameters of T. aestivum.
Total Chlorophyll a/b Ratio
The total chlorophyll a/b ratio is a key parameter in plant physiology and photosynthesis research, providing insights into the efficiency of light-harvesting pigments in chloroplasts. Chlorophyll a and b are essential pigments responsible for capturing light energy during photosynthesis. Researchers commonly determine this ratio through spectrophotometric analysis, measuring the absorbance of chlorophyll extracts at specific wavelengths. A higher chlorophyll a/b ratio often indicates a plant’s adaptation to low-light environments, while a lower ratio suggests adaptation to high-light conditions. The total chlorophyll a/b ratio aids in assessing plant health, stress responses, and adaptation strategies. This parameter is valuable in agricultural and ecological studies, helping scientists optimize crop growth conditions and comprehend the dynamics of plant ecosystems. The estimation of chlorophyll a/b ratio content (mg/g) of T. aestivum was recorded during the vegetative phase (Fig. 1). The result showed that the maximum chlorophyll a/b ratio was found at a sufficient level of boron B20 (0.1919,7.004). While the minimum chlorophyll a/b ratio was found at the highest level of boron B60 (0.1216, 2.52) at P<0.05.
Soluble Leaf Protein Contents
The soluble leaf protein contents are a critical measure in plant biochemistry, providing valuable information about the plant’s nutritional status, stress response, and overall metabolic activity. Soluble proteins in leaves play crucial roles in various physiological processes, including enzymatic reactions, signal transduction, and defense mechanisms. This parameter is particularly relevant in agricultural and ecological studies, helping researchers understand the impact of environmental factors, such as nutrient availability and stress conditions, on plant protein metabolism. Monitoring changes in soluble leaf protein contents is essential for assessing plant health, identifying stressors, and optimizing cultivation practices. The protein content (mg/g) was assessed during the nutrition phase (Fig. 1). Protein contents of T. aestivum L. showed promotion under a sufficient amount of boron B30 (6.323). While reduction was recorded in the excess level of boron B60 (2.333) at P<0.05.
Proline Contents
Proline contents are a vital indicator in plant biochemistry, often used as a biomarker for stress responses and environmental adaptation. Proline is a non-essential amino acid that plays a significant role in osmoregulation and acts as a protective solute during various stress conditions, including drought, salinity, and extreme temperatures. The measurement of proline contents provides insights into the plant’s ability to cope with environmental challenges. This parameter is particularly relevant in agriculture, where understanding the stress resilience of crops is essential for improving yield and sustainability. The comparison of proline content (mg/g) was determined at the nutrient stage. The proline content of T. aestivum is significantly intense under sufficient boron stress (Fig. 1). The maximum increment showed that under boron excess, B30 (26.666) was significantly similar to B20 (25.636). While the minimum increment showed under toxic boron B60 (21.35) at P<0.05.
Soluble Sugar Contents
The soluble sugar contents are a crucial parameter in plant biochemistry, serving as indicators of energy storage, metabolism, and responses to environmental conditions. Soluble sugars, including glucose, fructose, and sucrose, play essential roles in providing energy for various cellular processes and act as signaling molecules in plants. The quantification of soluble sugar contents is fundamental for understanding plant metabolism, growth, and stress responses. The assessments of sugar content (mg/g) at the vegetative stage were made. The sugar content of Triticum aestivum shows a significant increment under sufficient boron stress Fig. 2a) The result demonstrates that the maximum sugar content was found for a low amount of boron in B30 (77.333), which was significantly similar to B20 (76.014). While the minimum sugar content was found for toxic boron B60 (71.85) at P<0.05.
Carotenoid Contents
The carotenoid contents represent a significant aspect of plant biochemistry and are integral to various physiological processes. Carotenoids are pigments that contribute to the coloration of plants and play essential roles in photosynthesis and photoprotection. Carotenoids have antioxidant properties, contributing to the plant’s defense against oxidative stress. The quantification of carotenoid contents is crucial for understanding plant health, nutritional quality, and responses to environmental factors. The estimation of carotenoid content (mg/g) was carried out at the nutrient stage (Fig. 2). The results of carotenoid contents in Triticum aestivum showed a reduction under excess concentrations of boron. Maximum carotenoid content was observed at a sufficient level of boron B20 (6.076). While the minimum carotenoid content was observed at an excess amount of boron, B60 (1.957) was significantly similar to B50 (2.150) at P<0.05.
Total Phenol Contents
The total phenol contents are a significant parameter in plant biochemistry, providing insights into the antioxidant capacity, stress response, and potential health benefits of plant extracts. Phenolic compounds, including flavonoids and tannins, contribute to the plant’s defense mechanisms against various stressors, such as pathogens and environmental challenges. The measurement of total phenol contents is crucial for assessing the overall phenolic antioxidant potential of plant samples. The assessments of phenol content (mg/g) at the vegetative stage were made. The phenol content of T. aestivum shows a significant increment under sufficient boron stress (Fig. 2). The result showed that the maximum phenol content was found for sufficient treatments, B30 (18.315) was significantly similar to B20 (17.295). While the minimum phenol content was found for toxic boron B60 (14.000) at P<0.05.
Estimation of Amino Acid Contents
The estimation of amino acid contents is a fundamental aspect of biochemical analysis, playing an essential role in understanding the composition and nutritional value of proteins. The accuracy of amino acid estimation is crucial for applications in fields such as nutrition, biochemistry, and food science. The study of amino acids in Triticum aestivum during the vegetative phase under boron was determined. The amino acid content of Triticum aestivum shows a significant increment under sufficient boron (Fig. 2). The result indicated that the total amino acid content in Tritium aestivum was high under a sufficient concentration of boron B30 (20.650) and was significantly similar to B20 (18.990). While low amino acid content was observed at a lacking concentration of boron, B0 (15.115) was significantly similar to B10 (14.50) at P<0.05.
Discussion
Boron (B) is an essential micronutrient for the normal growth and development of plants, which is required for the proper maintenance of the physiological and biochemical processes of the plants. Their deficiency or excess affects these physiological and biochemical processes and is hence responsible for the decline in plant growth and productivity. Boron is supplied as a fertilizer in those areas where boron is lower in concentration, but high concentrations of boron can also be poisonous to plants [16]. The results of current studies show that out of the various concentrations of B, (50 mg/kg) was moderately toxic, while (60 mg/kg) generated high toxicity and induced a B stress response to confer tolerance in wheat. Moreover, a possible mechanism of B toxicity response in wheat is suggested. The biochemical result showed that the chlorophyll “a” and chlorophyll “b” contents were increased with a sufficient amount of boron (20 mg/kg) as compared to excess and deficient amounts of boron. These results are parallel with [17] observed that photosynthetic pigments (Chlorophyll “a” and chlorophyll “b”) contents were increased with a lower concentration of boron (4 µg/g) as compared to higher applied doses of boron. [18] observed a decrease in carotenoid, chlorophyll a, b, and total chlorophyll contents in boron deficient and boron excess treatments in comparison to boron sufficient treatments. [19] observed a reduction in carotenoid and chlorophyll contents at higher doses of boron (100, 300, and 500 μmol/l) in pear plants. A high concentration of boron decreased the levels of chlorophyll a, chlorophyll b, and carotenoid contents [20]. The present studies also indicate that a reduction in protein contents was observed at deficient and excess boron concentrations (B0, B50, and B60) and an increase at sufficient boron concentrations (B30). A similar result was reported by [20], who noted that the minimum protein contents at a lower dose of boron (4μg/g) and the maximum protein contents a at sufficient dose of boron (32μg/g) in wheat plants. [21] studied the protein profiles of barley in response to a higher concentration of boron. Proline is synthesized during nitrogen metabolism, functions as a protectant, and maintains cellular homeostasis [22-24] explored the boron-induced impacts on photosynthesis, growth, and the antioxidant system under various boron levels (0, 10, 20, 30, 40, 50, and 60mg/kg) in two varieties of Brassica juncea. The B treatments (20, 30, 40, 50, or 60 mg/kg) significantly increased the proline and activity of antioxidant enzymes (CAT, SOD, and POX) in both varieties. The studies in [25] support and are in accordance with the present investigation. In our study, an increase in the accumulation of proline content increase at sufficient boron concentrations (B20 and B30 mg/kg) may be due to increased proline biosynthesis and protein breakdown or decreased breakdown of proline. The current studies also indicated a variation in the sugar content at various concentrations of boron. The decrease in sugar content was observed at toxic boron concentrations (B60) and increased at sufficient boron concentrations (30 mg/kg). These results are similar to the views of [26-28]. In present studies, an increase in the soluble sugar content at sufficient soil boron applications indicates plants’ adaptive response to boron stress for efficient translocation of boron for their active exclusion from the roots to the soil [29]. The maximum increase in carotenoid contents was observed at a sufficient level of boron (20 mg/kg). Beyond this concentration, carotenoid contents started decreasing at higher concentrations, of boron. A decrease in carotenoid contents has been reported by [30], who observed a decrease in chlorophyll and carotenoid contents at higher doses of boron (100, 300, and 500μmol/l) in pear plants. The decreased levels of chlorophyll a, chlorophyll b, and carotenoid contents were observed as boron concentration increased [31]. A reduction in carotenoid contents was observed under boron stress conditions (10 and 20 mg L-1 nutrient solution) in Cucurbita pepo, while no significant difference in carotenoid contents was observed in Cucumis sativus. The study examined the effects of boron toxicity on two genotypes of tomato (cv. Kosaco and cv. Josefina). Under 0.5- and 2-mM application of boron, the leaves of cv. Josefina showed a maximum carotenoid concentration, whereas this did not occur in cv. Kosaco. Phenolic compounds are the markers of stress in plants. In the present investigations, phenolic accumulation was observed at sufficient amounts of boron concentrations (30 mg/kg). The same result was reported by [32] and [33], who noticed a remarkable increase in leaf total phenolic concentration as a tolerance measure to cope with boron sufficiency. Our result showed that the maximum concentration of amino acid content was reported at a sufficient amount of boron (20 and 30 mg/kg), which was significantly similar to [34]. This indicates that the boron application had a positive effect on the amino acid content of wheat plants.
Conclusion
This work concluded that among all the micronutrients, boron’s role is remarkable not only with its chemical properties but also with its role in plants. It is required for the translocation of photosynthates from source to sink and hence helps in improving the yield and quality of fruit crops. In boron-deficient soils, boron application in the form of borax or any other boron fertilizer helps in reducing deficiency – disorders like internal necrosis, dieback, fruit hardening, chlorosis, rosette, fruit cracking, etc. in fruit crops. The amount of boron present or available to plants depends upon different factors like soil pH, texture, clay content, etc., which need to be considered during boron application. From the above discussion, it can be concluded that both B deficiency and toxicity alter the physiology and biochemistry of plants. It causes inhibition of root growth, plant height, plant biomass, and finally plant growth. Moreover, biochemical content also decreased under B deficiency and excess levels. The biochemical contents are maximum at sufficient concentrations for B20 and B30 treatment, and the plant grows well and is healthy at this level. Therefore, growing B tolerant crops may be the only possible solution to boron toxicity and deficiency.

