

Introduction
Pulses are considered an important protein source with high biological value. They serve as an excellent complement to cereals, enhancing the overall protein content in vegetarian diets. Nonetheless, the decline in pulse consumption in India has contributed to an alarming rise in malnutrition, resulting in inadequate protein intake, as indicated by household consumption surveys [1]. As per the Global Hunger Index report, 16.3% of the world’s undernourished population lives in India [2]. Malnutrition affects one in three people worldwide, potentially due to hidden hunger or micronutrient deficiency [3]. In the world’s total pulses area and production, India accounts for about 38% of the area and 28% of the production, respectively, making it the largest producer and consumer in the world [4]. Recent studies have shown positive correlations between a decline in pulse production and a high level of malnutrition [5, 6]. It is estimated that there will be a sharp rise in pulse demand by 2050, necessitating an annual production growth of 2.2% [7].
Chickpeas (Cicer arietinum L.) rank third worldwide in rabi-seasoned pulse crops and cover approximately 14.84 million hectares in area, with productivity around 15.08 million metric tons [8, 9]. India dominates the chickpea market, contributing to 70% of the total annual production [10]. The major chickpea-producing states in India are Maharashtra (25.97%), Madhya Pradesh (18.59%), Rajasthan (20.65%), Gujarat (10.10%), and Uttar Pradesh (5.64%) (IIPR, 2023). Enriched with total carbohydrates (64%), protein (23%), starch (47%), fat (5%), soluble sugar (6%), crude fiber (6%), and ash (3%), chickpeas have contributed immensely towards global food and nutritional security [11, 12]. As per the World Health Organization’s suggestions, chickpeas have gained recognition among nutritionists and food producers as a healthful plant-based dietary choice. This heightened awareness has led to a surge in global demand for chickpeas as a dietary staple. However, low productivity, shifting climates, and surging abiotic and biotic stresses constrain them from fulfilling the burgeoning population demand. Besides, proposed policies that support staple crop production, like fertilizer subsidies, credits, and irrigation facilities, are the biggest obstacles to achieving pulse self-sufficiency [13]. Therefore, further breakthroughs and yield resilience are urgent in the current global scenario.
Among various agricultural concerns, water constraint or drought stress stands out as a significant limiting factor for low productivity, accounting for 60- 70% of annual yield losses in rain-fed areas [14, 15]. Drought can affect crop germination, growth phases, and yield by affecting morphological (e.g., seedling length and biomass), physiological (e.g., relative water content), biochemical (e.g., amylase, protease, and lipase activities), and molecular (e.g., stress proteins, aquaporins, and dehydrins) characteristics [16]. Specifically, during reproductive stages, water stress affects grain development, number of grains per panicle, grain weight, and other yield-related traits, resulting in a significant decrease in productivity and final production quality [17-21]. Generally, plants are self-reliant in adjusting themselves at morphological, physiological, biochemical, and molecular levels to some extent under unfavorable climatic conditions. Still, these natural mechanisms are insufficient to produce the desired results [22, 23].
To manage these drought stress challenges, efficient, simple, and manageable technologies/approaches need to be considered to improve holistic crop growth and development. One such novel strategy is the simple and efficient hydration approach to seeds to reduce the considerable yield losses under water-limited conditions. The seed priming approach is an effective technology in which seeds undergo a physiological process of alternate regulated hydration and drying, resulting in an improved and enhanced pre-germinative metabolic process and faster germination [24]. This hydration technique can utilize various natural and synthetic materials to induce a seed state known as the “primed state”. During this phase, various cellular reactions occur, including the activation of enzymes and genes such as late embryogenesis abundant (LEAs) before germination, in order to respond to or develop resistance against abiotic stresses [25]. Among the methods used for seed priming, nutria-priming, and phytohormonal priming are win-win priming techniques in the agriculture sector. Zinc, a vital component of many biomolecules such as proteins, lipids, and auxin co-factors, catalyzes essential physiological reactions, including nucleic acid and carbon metabolism in plants. Furthermore, Zn plays a crucial role as a stimulator of carbonic anhydrase and aldolase in plants. Several studies revealed that applying zinc can enhance crop yield and quality by modulating drought tolerance in various crops such as wheat, red cabbage, sunflower, and tomato [26-28]. Boron (B) as a micronutrient also has a prominent role in the reproductive growth of crops, affecting pollen fertility, seed development, the setting of pods, and ultimately grain yield [29]. Besides, B maintains membrane integrity, stabilizes plant cell walls, facilitates sugar transport, and enhances plant calcium and nitrogen utilization [29, 30]. The aforementioned physiological roles of Zn and B in vegetative and reproductive growth suggest that the nutria-priming options of Zn and B under drought conditions are an effective strategy for improving the antioxidant activities and biochemical parameters in chickpeas. Moreover, salicylic acid (SA) plays a critical role in reducing the impact of environmental stress by regulating the antioxidant defense system. This involves activating the expression of genes and biosynthetic enzymes responsive to both biotic and abiotic stress. SA also promotes the up-regulation of synthesis for heat shock proteins, chaperones, and dehydrin-like proteins, resulting in decreased reactive oxygen species (ROS) production in photosynthetically active tissues [31]. Enhancement in stomatal movement, transpiration rates, and photosynthetic rates has been documented in various studies following the exogenous application of SA either as a foliar spray or through seed priming techniques [32].
The impact of nutria (Zn and B) and hormonal priming (SA) for improving drought tolerance in chickpeas are limited. The present investigation aims to assess the possible impacts of seed priming techniques with zinc sulfate (ZnSO4), boron (B), and salicylic acid (SA) on ameliorating the injurious effects of water-limiting stress by evaluating various agromorphological and physio-biochemical parameters in chickpea under critical growth stages.
Materials and Methods
Plant Material and Growth Conditions
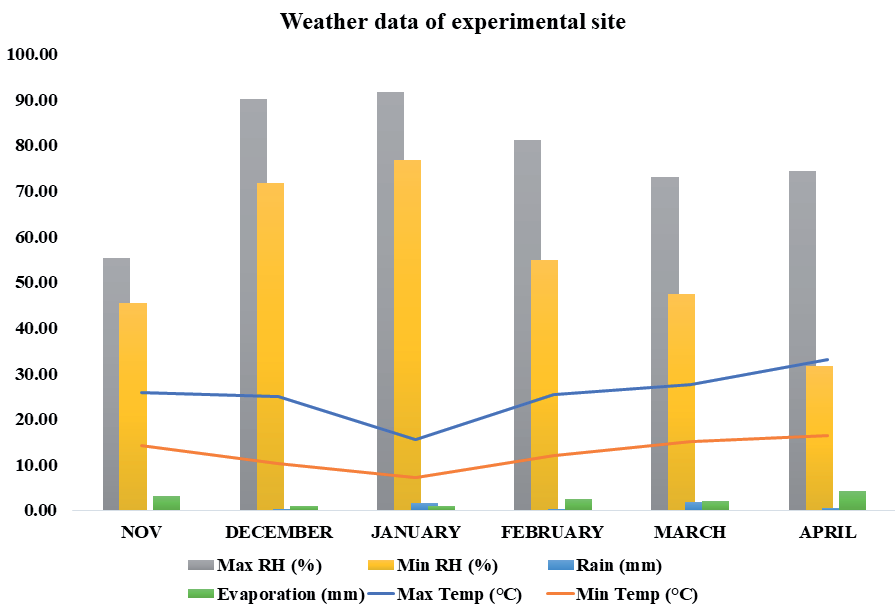
The current investigation was undertaken at Lovely Professional University, Punjab, India, on drought-susceptible chickpea (Cicer arietinum L.) genotype GNG 469. The investigation was to assess the possible impacts of seed priming techniques with zinc sulfate (ZnSO4), boron (B), and salicylic acid (SA) in ameliorating the injurious effects of water-limiting stress by evaluating various agromorphological and physio-biochemical parameters in chickpea under critical growth stages. Soil samples were collected and analyzed to determine available NPK, organic carbon (OC), and various chemical properties of the experimental site (Table 1). Mean monthly weather parameters of the chickpea-growing site are presented in Fig. 1. Current research was conducted in a randomized block design (RBD) with three replications for both primed and unprimed treatments. The complete descriptions of treatments were T0: control/hydroprimed, T1: SA-primed seeds, T2: boron-primed seeds, and T3: ZnSO4-primed seeds (0.5%) under normal vs. water-limiting stress conditions. The observations were recorded under various critical stages (40, 80, and 120 DAS).
Seed Priming
The seeds underwent thorough surface sterilization using a solution of mercuric chloride (0.01%) for 5 min, followed by rinsing with distilled water thrice before undertaking the priming treatments. Furthermore, seeds were subjected to two priming strategies, i.e., nutria-priming and hormonal priming. Two effective micronutrients, Zn and B, were used for nutria-priming, where the solutions were prepared and the seeds were dipped for 12 h, followed by alternate drying. A similar procedure was also followed for hormonal priming with SA. Drought stress was induced by withholding irrigation for at least 10 days during critical growth stages, encompassing both vegetative and reproductive phases.
Chemical Analysis of Soil at the Pre-experiment Stage
A standard protocol was followed to estimate available N, P, and K in soil [33-35], whereas organic C, pH, and EC were estimated through the Walkley and Black method [36], a glass electrode pH meter [36], and Method No.4 USDA Handbook No.16 [37], respectively.
Physiological and Biochemical Parameters Analysis
Estimation of Total Chlorophyll Content
A standard protocol was followed to estimate total chlorophyll content [38] in the first fully expanded green leaves. The 0.5 g of leaves were crushed in a mortar and pestle using 5 mL of acetone solution (80%), and absorbance was read at 645 and 663 nm in a spectrophotometer (Techcomp UV 2600).
Estimation of Proline Content
Free proline content was estimated through a standard procedure [39]. A leaf sample weighing 0.5 g was homogenized with sulfosalicylic acid (3%). The 2 mL of glacial acetic acid and ninhydrin reagent were added to the 2 mL extract, followed by boiling in a water bath. The reaction mixture was separated by adding 6 mL of toluene in a separating funnel, and absorbance was read at 520 nm in the spectrophotometer against a toluene blank.
Estimation of Malondialdehyde (MDA) Content
MDA is an important parameter to estimate lipid peroxidation level and was estimated through the procedure discussed in reference [40]. A leaf sample weighing 0.5 g was homogenized in 0.1% tricarboxylic acid (TCA), followed by centrifugation of the sample. To 1.0 mL of the supernatant, 4.0 mL of a solution containing 0.5% thiobarbituric acid (TBA) and 20% trichloroacetic acid (TCA) was added. The mixture was then heated at 95°C for 30 min and promptly cooled in an ice bath. Subsequently, the absorbance was measured at 532 nm.
Table 1.
Chemical analysis of soil at the pre-experiment stage.
Estimation of the Membrane Stability Index (MSI)
Fresh leaf material was placed in a glass beaker to determine the conductivity of the solution (C1) at 30ºC for 1 h. Subsequently, the samples were boiled for 2 min, and the conductivity (C2) was measured again. The membrane stability index (MSI) was calculated using the prescribed method [41]:
MSI (%) = [l - (C1/C2)] x 100
Estimation of Total Phenolic Content (TPC)
Total phenolic content was quantified according to the prescribed method in reference [42]. One g of the leaf sample was macerated with 15 mL of methanol (50%), followed by a volume makeup to 50 mL in a volumetric flask. One mL of the sample extract was mixed with 4 mL of 20% (w/v) Na2CO3 and 10 mL of distilled water in a volumetric flask, and the volume was adjusted to 25 mL. The mixture was agitated and left for 30 min at room temperature. Subsequently, the absorbance of the sample was measured at 765 nm. Quantification was carried out using a standard curve of gallic acid.
Estimation of Ascorbate Peroxidase (APX)
(EC 1.11.1.11)
The ascorbate peroxidase (APX) enzyme extract was analyzed using the method described in reference [43]. To prepare the extract, 100 mg of leaf sample was homogenized with 1 mL of extraction buffer consisting of 0.1 M phosphate buffer (pH 7.5) containing 0.5 mM ethylenediaminetetraacetic acid (EDTA) and 1 mM ascorbic acid. After centrifugation at 10,000 g for 10 min at 4ºC, the supernatant was collected as the enzyme source. The reaction mixture, totaling 3 mL, comprised 1.5 mL of 100 mM buffer, 50 mM ascorbic acid, 0.1 mM EDTA, 0.1 mM H2O2, 0.2 mL of enzyme, and 0.6 mL of water. The decrease in absorbance over 30 seconds was measured at 290 nm using a UV-visible spectrophotometer. Enzyme activity was calculated as ascorbic acid oxidized per minute, per mg protein, or per gram fresh weight.
Estimation of Catalase Activity (CAT)
(EC 1.11.1.6)
The enzyme was assayed following the standard protocol [44]. Leaf samples (0.1 g) were macerated in 5 mL of 0.1 M phosphate buffer, followed by centrifugation. The enzyme activity was assessed using a mixture comprising 2.6 mL of 0.1 M phosphate buffer, 0.1 mL of enzyme extract, and 0.1 mL of 1% H2O2. Absorbance changes at 240 nm (δ A240) were recorded at 15-sec intervals over a period of 2 min.
Statistical Analysis
Descriptive statistics and cluster analysis of the assessed parameters were calculated using Minitab v 19.0 software [45]. Analysis of variance (ANOVA) based on a generalized linear model was also carried out using Minitab v 19.0 software to estimate the significant effects of seed priming treatments under normal vs. water-limiting stress at vegetative and reproductive growth stages and all their possible interactions (stage X stress and stage X seed priming treatments) for evaluated traits. Furthermore, the R package was used to do principal component analysis.
Results
Variance Analysis for the Estimated Parameters
ANOVA revealed highly significant effects of studied growth stages, i.e., vegetative and reproductive, water-limiting stress, and seed-priming treatments for almost all the evaluated parameters (Table 2). Growth stages were found to be non-significant for MSI, LP, proline, and CAT, while seed priming treatments had non-significant effects for TPCL and CAT (Table 2). Stage X stress interaction was found to be significant only for PH, TNBP, TCC, and proline; stage X treatment was non-significant, while stress X treatment was found significant for TPCL, CAT, APX, LP, and yield attributes and non-significant for all the estimated parameters.
Mean Variability of Agronomic Parameters
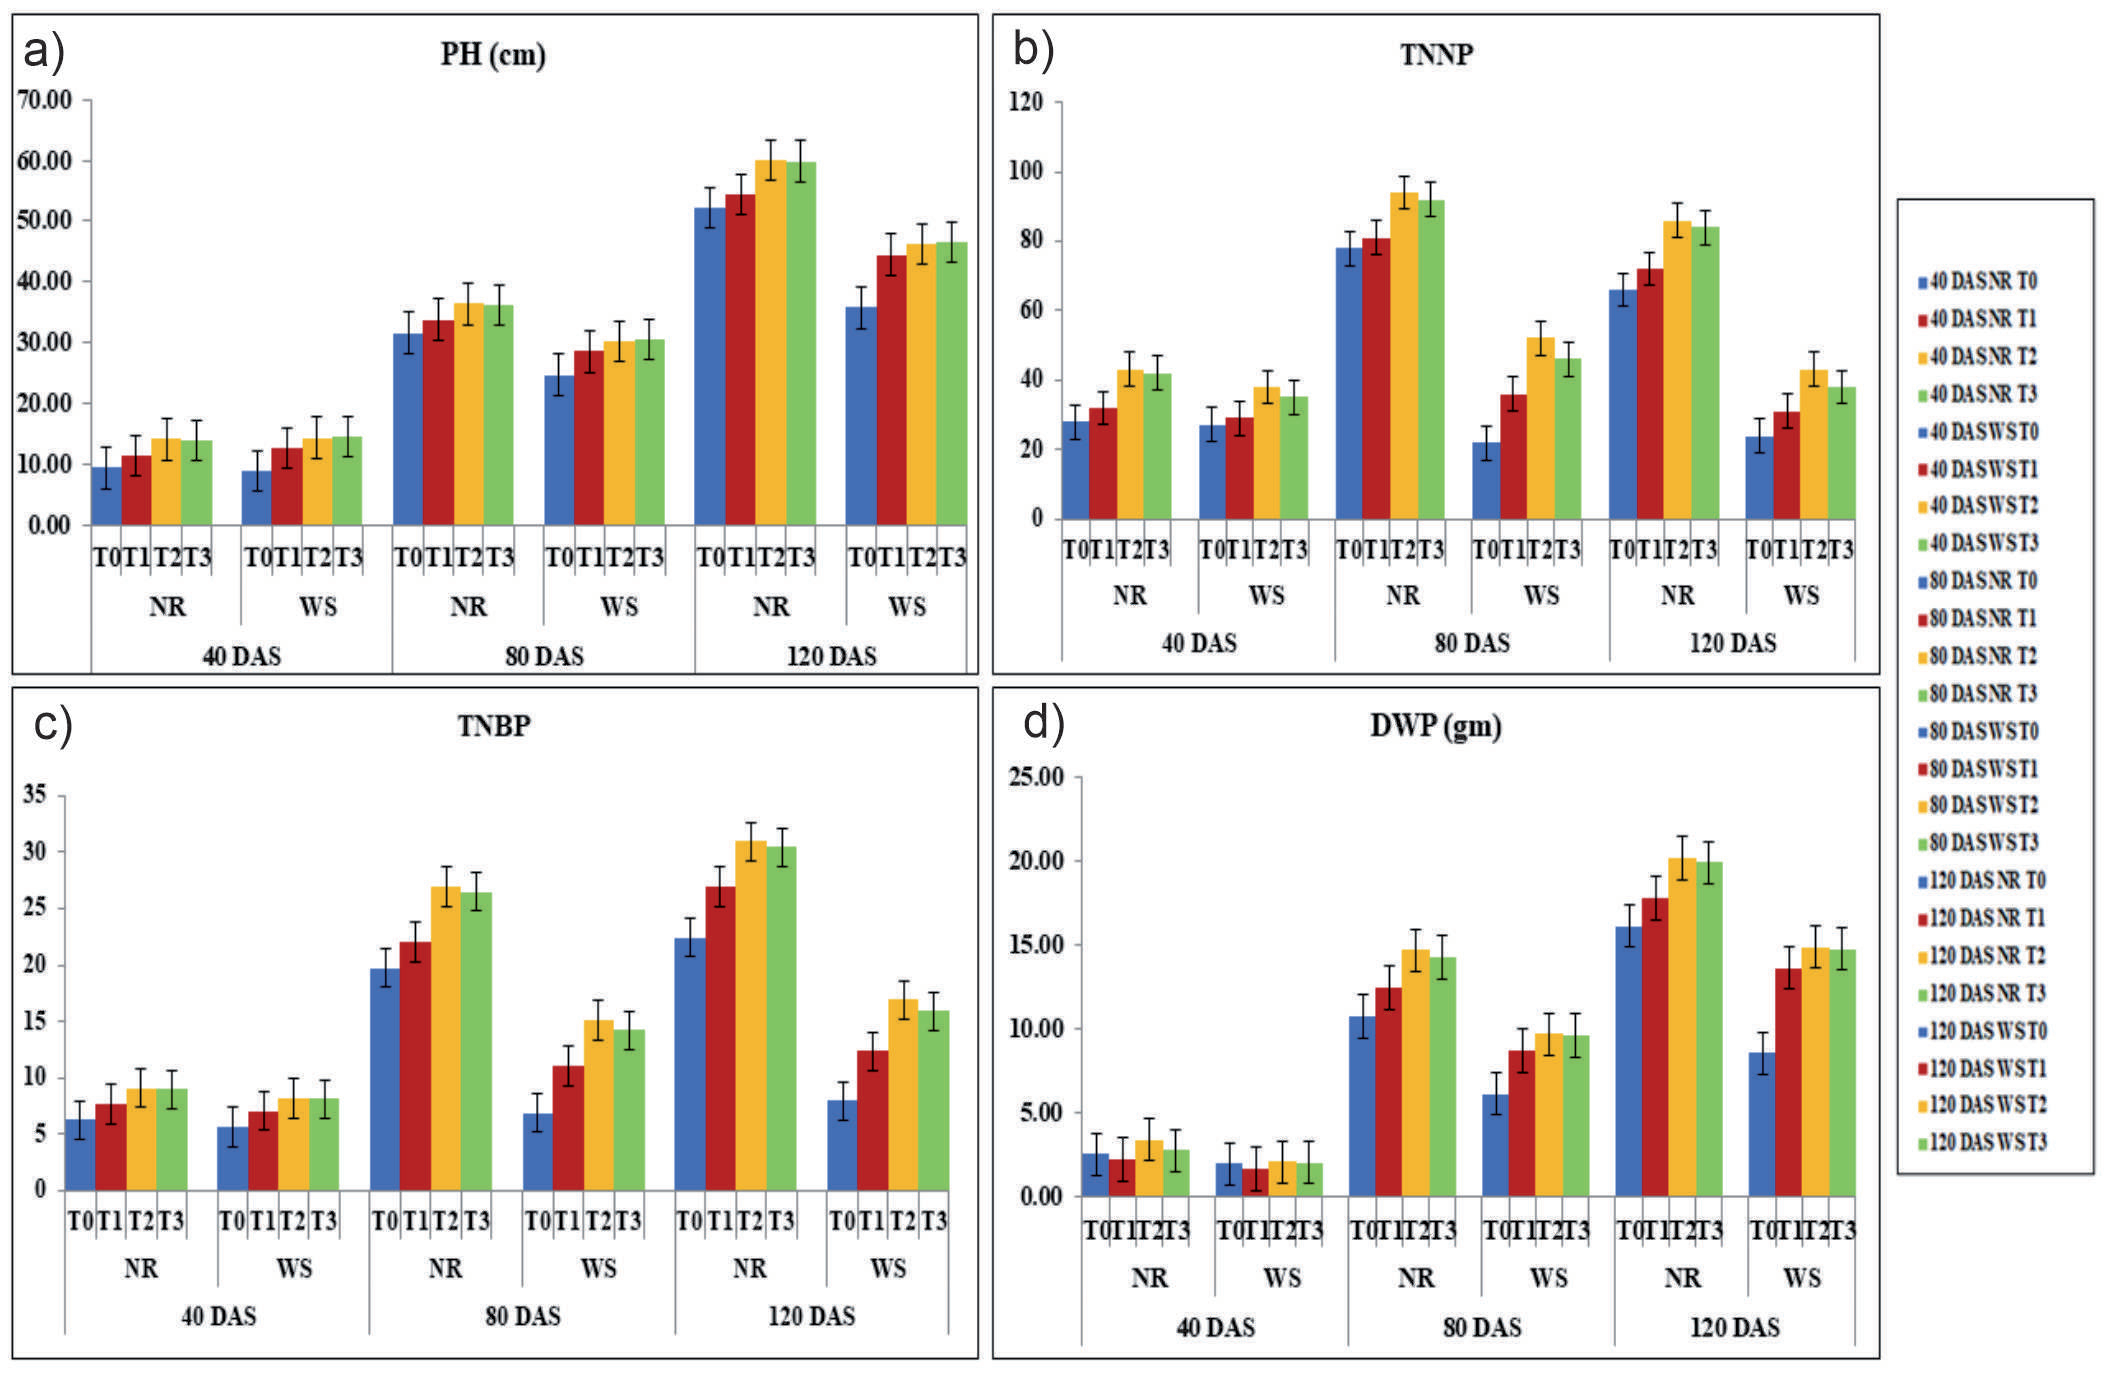
Water-limited stress significantly (p<0.05) interrupted the chickpea’s parameters of growth in terms of plant height (PH), total dry weight plant−1 (DWP), total number of branches plant−1 (TNBP), and total number of nodules plant−1 (TNNP) at critical growth stages when compared with the normal priming treatments (Fig. 2). However, applying different seed priming treatments (B, Zn, and SA) revealed the amelioration effects on various chickpea parameters of growth. Growth parameters were significantly improved through boron priming treatment, followed by Zn and SA among water-limited stress treatments. Among the normal priming treatments (soil and water conditions), both Zn and B priming treatments are found statistically at par with the control, whereas the SA priming indicated some significant differences in the data, both in water-stressed and normal priming treatments. Under water-stressed conditions, boron priming treatment increased the plant height by 13.4%, 5.6%, and 3.8%; and the total number of branches per plant by 15.4%, 36.8%, and 36.9%; the total number of nodules per plant by 31%, 44.4%, and 38.7%; the total dry weight per plant by 27.2%, 10.9%, and 8.91% at 40, 80, and 120 DAS, respectively, as compared to the values of SA-primed seeds under water stress milieu. In general, the best priming treatment of boron clarifies the maximum growth parameters under water stress conditions, whereas similar results were also revealed in normal irrigated treatments compared to SA and Zn treatments.
Table 2.
Analysis of variance for the estimated traits with varying seed priming treatments at varying growth stages under normal vs. water-limiting stress.
Fig. 2.
Agronomic parameters at varying seed priming treatments and various growth stages under normal vs. water-limiting stress conditions. Data are presented as Mean±S.E. The letters CO: control; NR: normal; WS: water limiting stress; T0: control/hydroprimed; T1: SA primed seed; T2: Boron primed seeds; T3: ZnSO4 primed seeds (0.5%); PH: plant height; TNNP: total number of nodules plant−1; TNBP: total number of branches plant−1; DWP: dry weight plant−1.
Mean Variability of Physiological Parameters
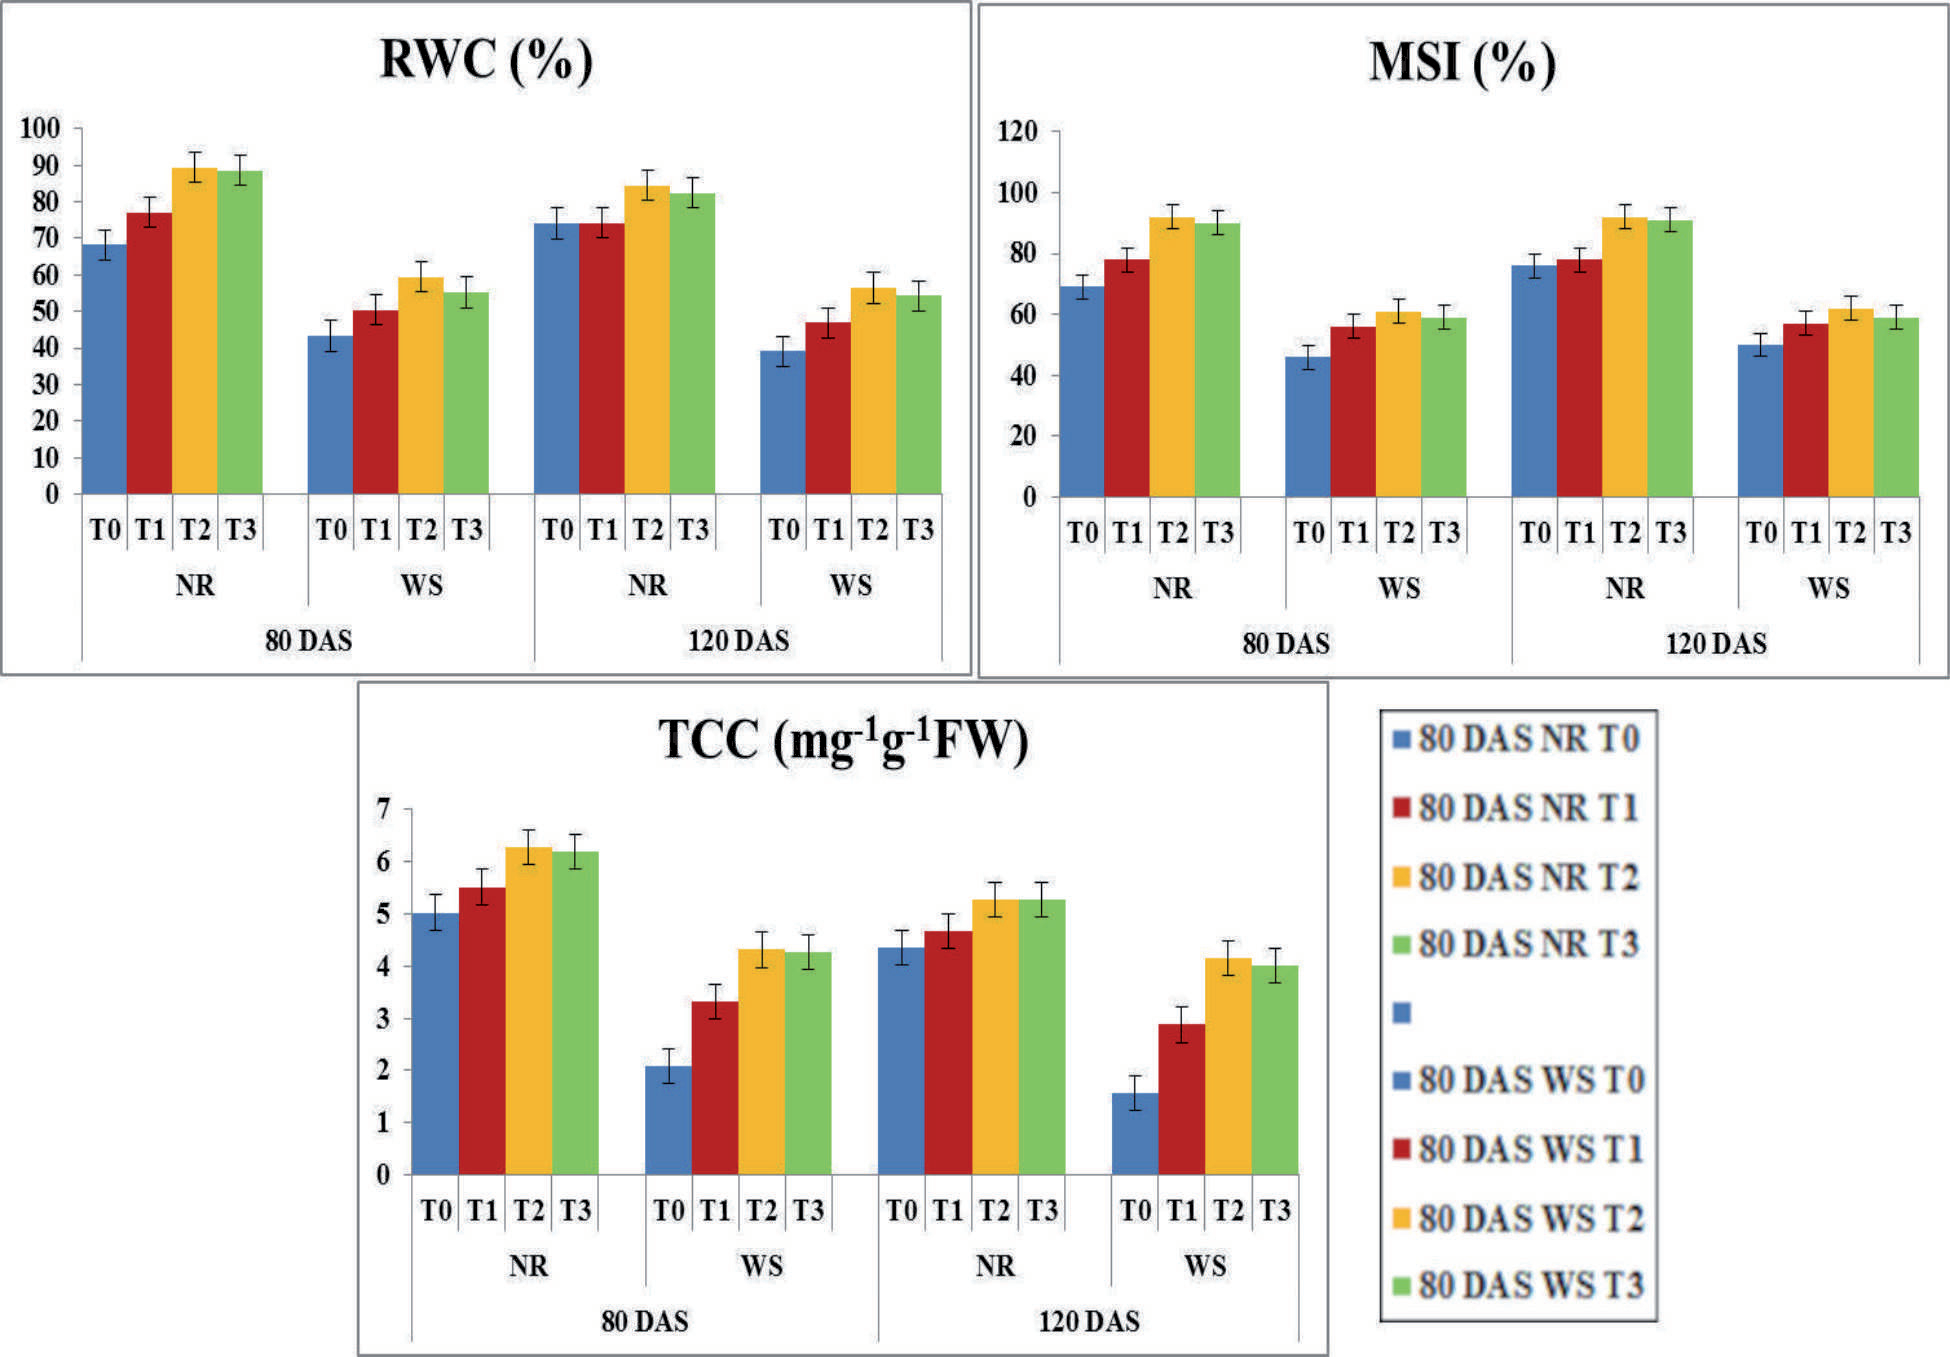
Drought stress statistically (p<0.05) reduced the total chlorophyll content (TCC), relative water content (RWC), and membrane stability index (MSI) (Fig. 3). However, the results revealed the mitigation effects of water stress by B and Zn priming treatments on physiological parameters at critical growth stages (80 and 120 DAS). The data revealed that, among the water stress treatments, TCC, RWC, and MSI were substantially enhanced in leaves of boron-primed plants, whereas minimum values were observed in SA-primed plants. Physiological parameters were statistically influenced in B-treated plants, followed by Zn-treated plants, under both irrigated and water-stressed treatments. Under water-stressed conditions, boron-primed seeds increased the TCC by 29.8% and 44.5%, RWC by 17.9% and 20.4%, and MSI by 8.9% and 8.7%, respectively, as compared to the values of the SA priming treatments at 80 and 120 DAS. Overall, the maximum total chlorophyll content of RWC and MSI was noted in the B-treated plants, followed by Zn priming treatments under both priming conditions (irrigated and water stress conditions).
Mean Variability of Biochemical Parameters and Antioxidant Enzyme Activities
Water stress significantly (p<0.05) augmented the lipid peroxidation and elicited the levels of free proline content, total phenolic content, and activities of APX and CAT to some extent in stressed plants (Fig. 4). However, with the application of priming agents B and Zn, biochemical parameters and antioxidant enzyme activities were significantly increased under water-stressed treatments. Moreover, the level of MDA was significantly reduced in B-primed treatments followed by Zn under water-stressed plants compared with the control. Unprimed treatments are at par in antioxidant enzyme activities (CAT and APX) values, whereas priming treatments under water-stressed conditions had higher values. The total proline and phenolic content was also higher in water-stressed plants with priming treatments than in normal irrigated plants. However, the highest values were revealed in boron-primed plants, followed by Zn under stressed conditions. SA treatments revealed the lowest values in both the irrigated and water-stressed plants. Under the water-stressed B-primed condition, the concerned priming treatments improved the activities of APX by 18.7% and 14%, CAT by 23.6% and 16.1%, total phenolic content by 40% and 16.3%, and free proline content by 25.3% and 24.8%, but reduced the MDA content by 25% and 22% at two critical growth stages (80 and 120 DAS) as compared to the values of water-stressed SA priming treatments. Results showed that B priming treatments were more effective, followed by Zn and SA under both irrigated and water-stressed conditions.
Fig. 3.
Physiological parameters at varying seed priming treatments and various growth stages under normal vs. water-limiting stress conditions. Data are presented as Mean±S.E. The letters CO: control; NR: normal; WS: water-limiting stress; T0: control/hydroprimed; T1: SA-primed seed; T2: boron-primed seeds; T3: ZnSO4-primed seeds (0.5%); RWC: relative water content; MSI: membrane stability index; TCC: total chlorophyll content.
Mean Variability of Yield and Yield-related Attributes
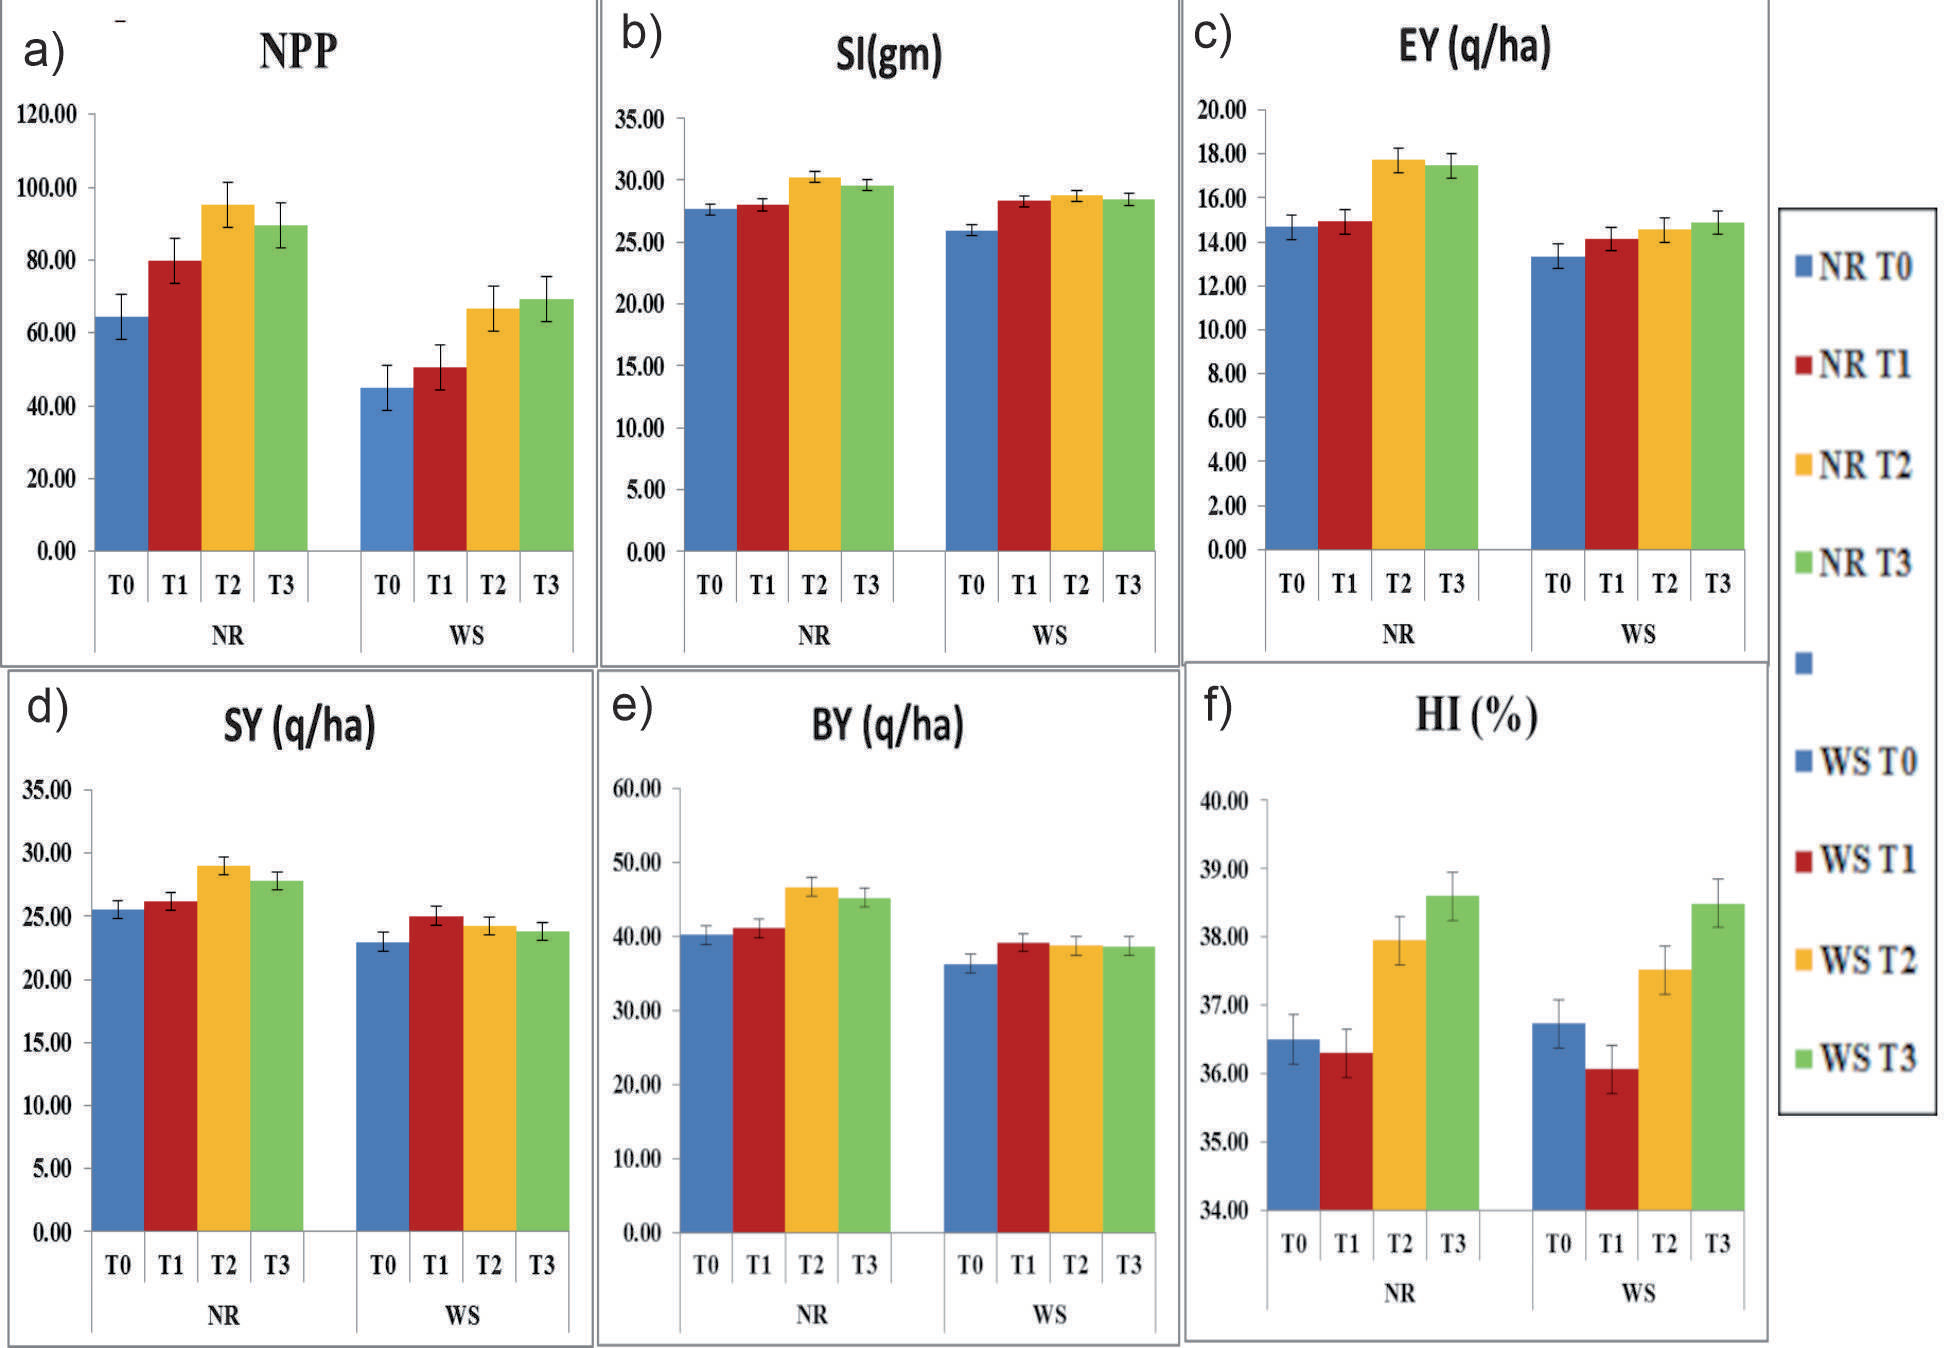
Results revealed that water stress significantly reduced the yield and yield-attributing characters in chickpea (Fig. 5). However, priming with micronutrients and phytohormones had amelioration effects on the number of pods per plant-1 (NPP), seed index (SI), economic yield (EY), stover yield (SY), biological yield (BY), and harvest index (HI) under water stress conditions. The results indicated that the yield-attributing characters differed significantly among treatments, and the highest-yield attributing characters were recorded in individual boron-primed treatments, followed by single treatments of Zn and SA, whereas the lowest values were recorded in water-stressed treatments of SA. Different micronutrients statistically influenced chickpea yields in terms of SI, HI, and SY under limiting water stress conditions. Overall, the respective priming individual treatments increased HI, and the maximum was recorded in boron-primed plants, whereas the lowest was recorded in SA-primed treatments under water-limiting stress.
Multivariate Analysis
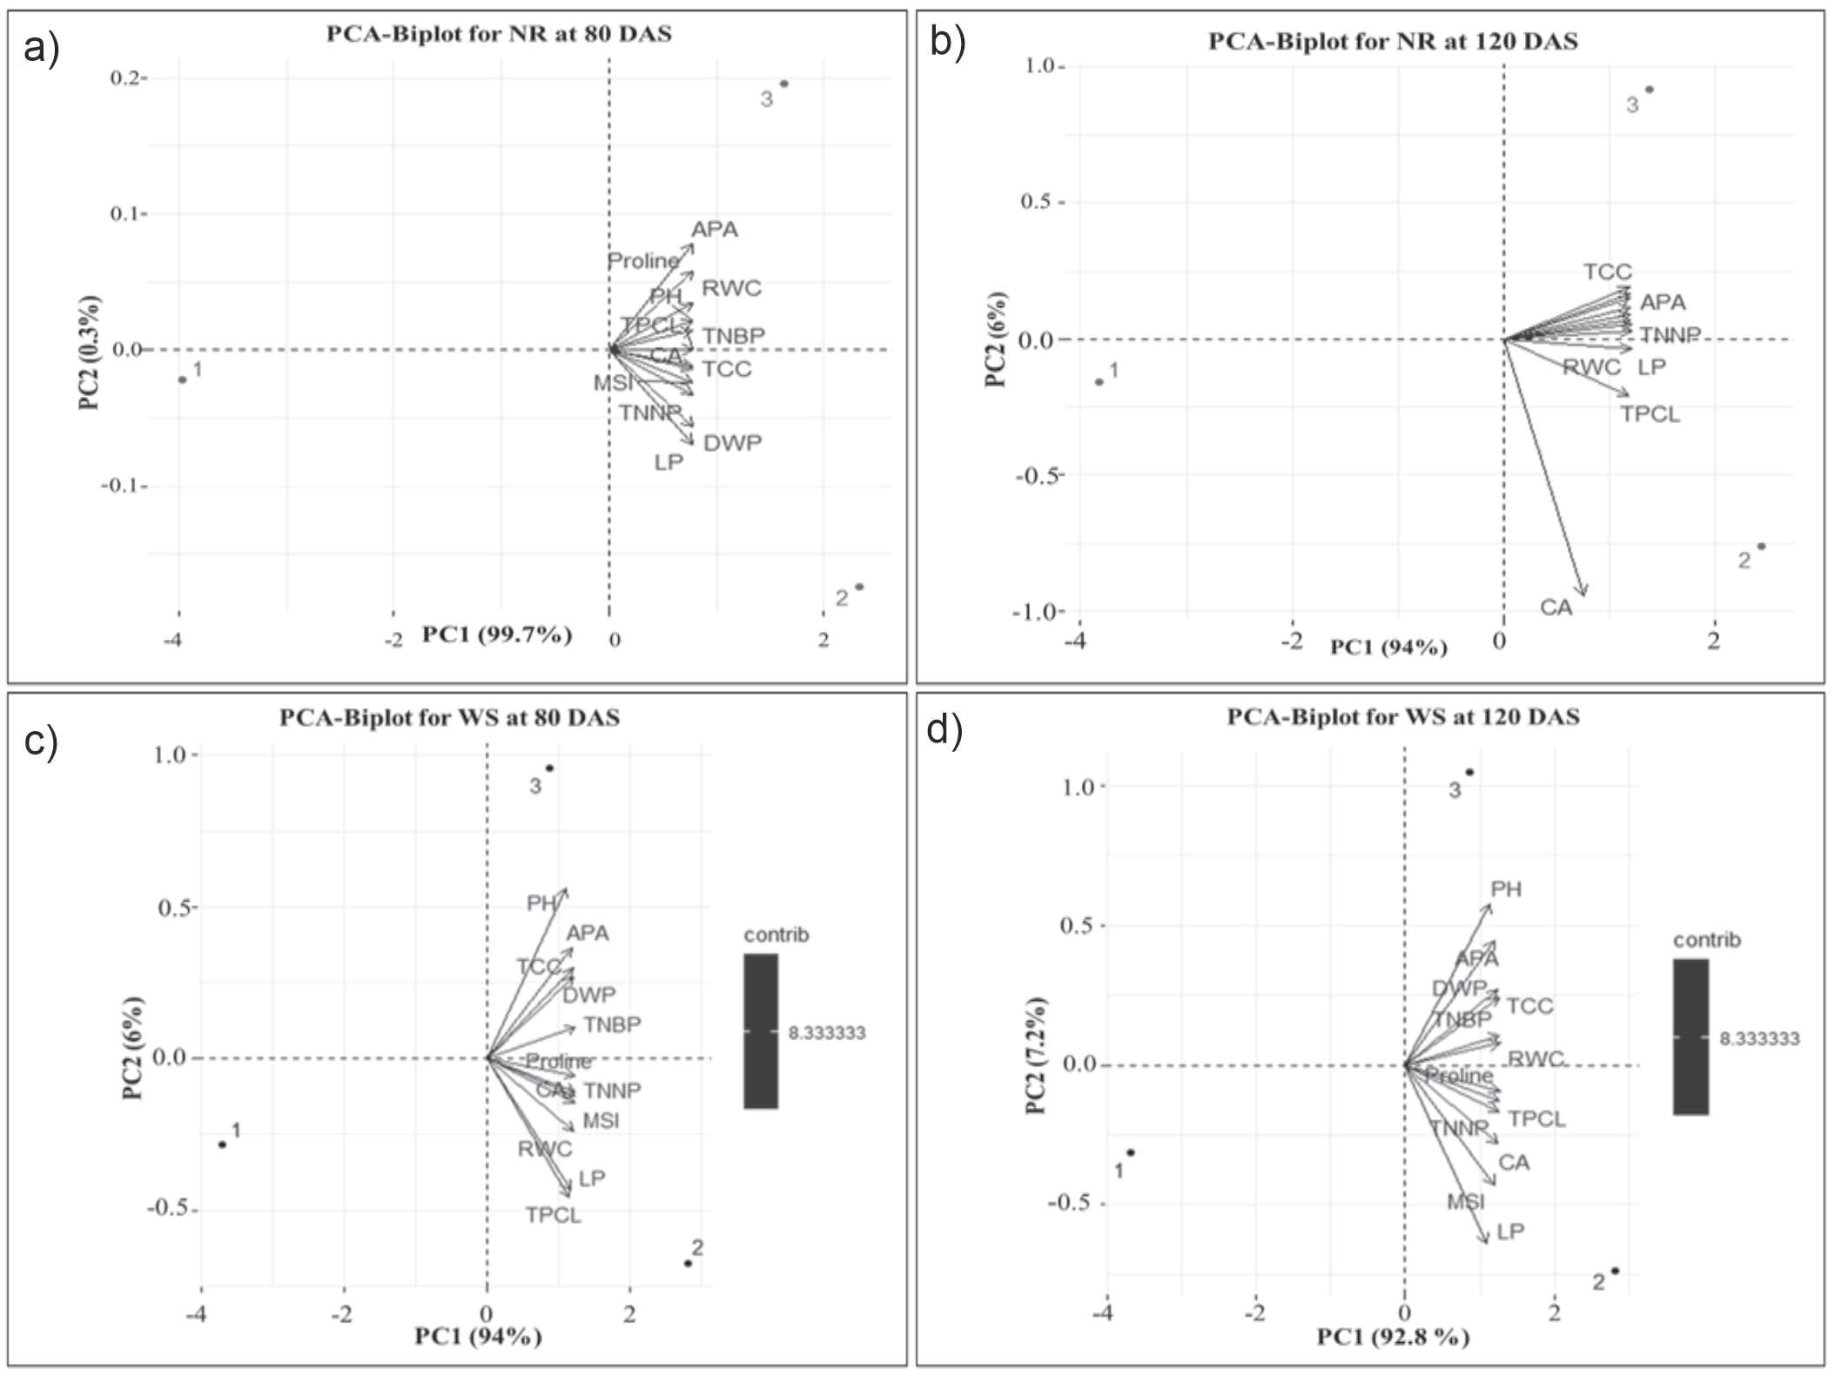
Multivariate analyses, such as cluster and principal component analysis (PCA), were used to define the group of traits that were significantly different from each other with different seed priming treatments under normal vs. stress conditions at vegetative and reproductive stages. Both PCA and cluster analysis revealed that under normal conditions, all traits were almost similar (two small clusters with > 99% similarity) at 80 DAS, while at 120 DAS, all traits were clustered together except for catalase activity (CAT). Under stress conditions, almost all the estimated traits were playing a significant role in adjusting drought stress with varying priming treatments at both 80 (two small clusters with > 80% similarity) and 120 DAS (two small clusters with > 75% similarity) (Fig. 6 and 7).
Fig. 4.
Biochemical parameters and antioxidant enzyme activities at varying seed priming treatments and various growth stages under normal vs. water-limiting stress conditions. Data are presented as Mean±S.E. The letters CO: control; NR: normal; WS: water-limiting stress; T0: control/hydroprimed; T1: SA-primed seed; T2: boron-primed seeds; T3: ZnSO4-primed seeds (0.5%); LP: lipid peroxidation; TPCL: total phenolic contents; CAT: catalase activity; APX: ascorbate peroxidase activity.
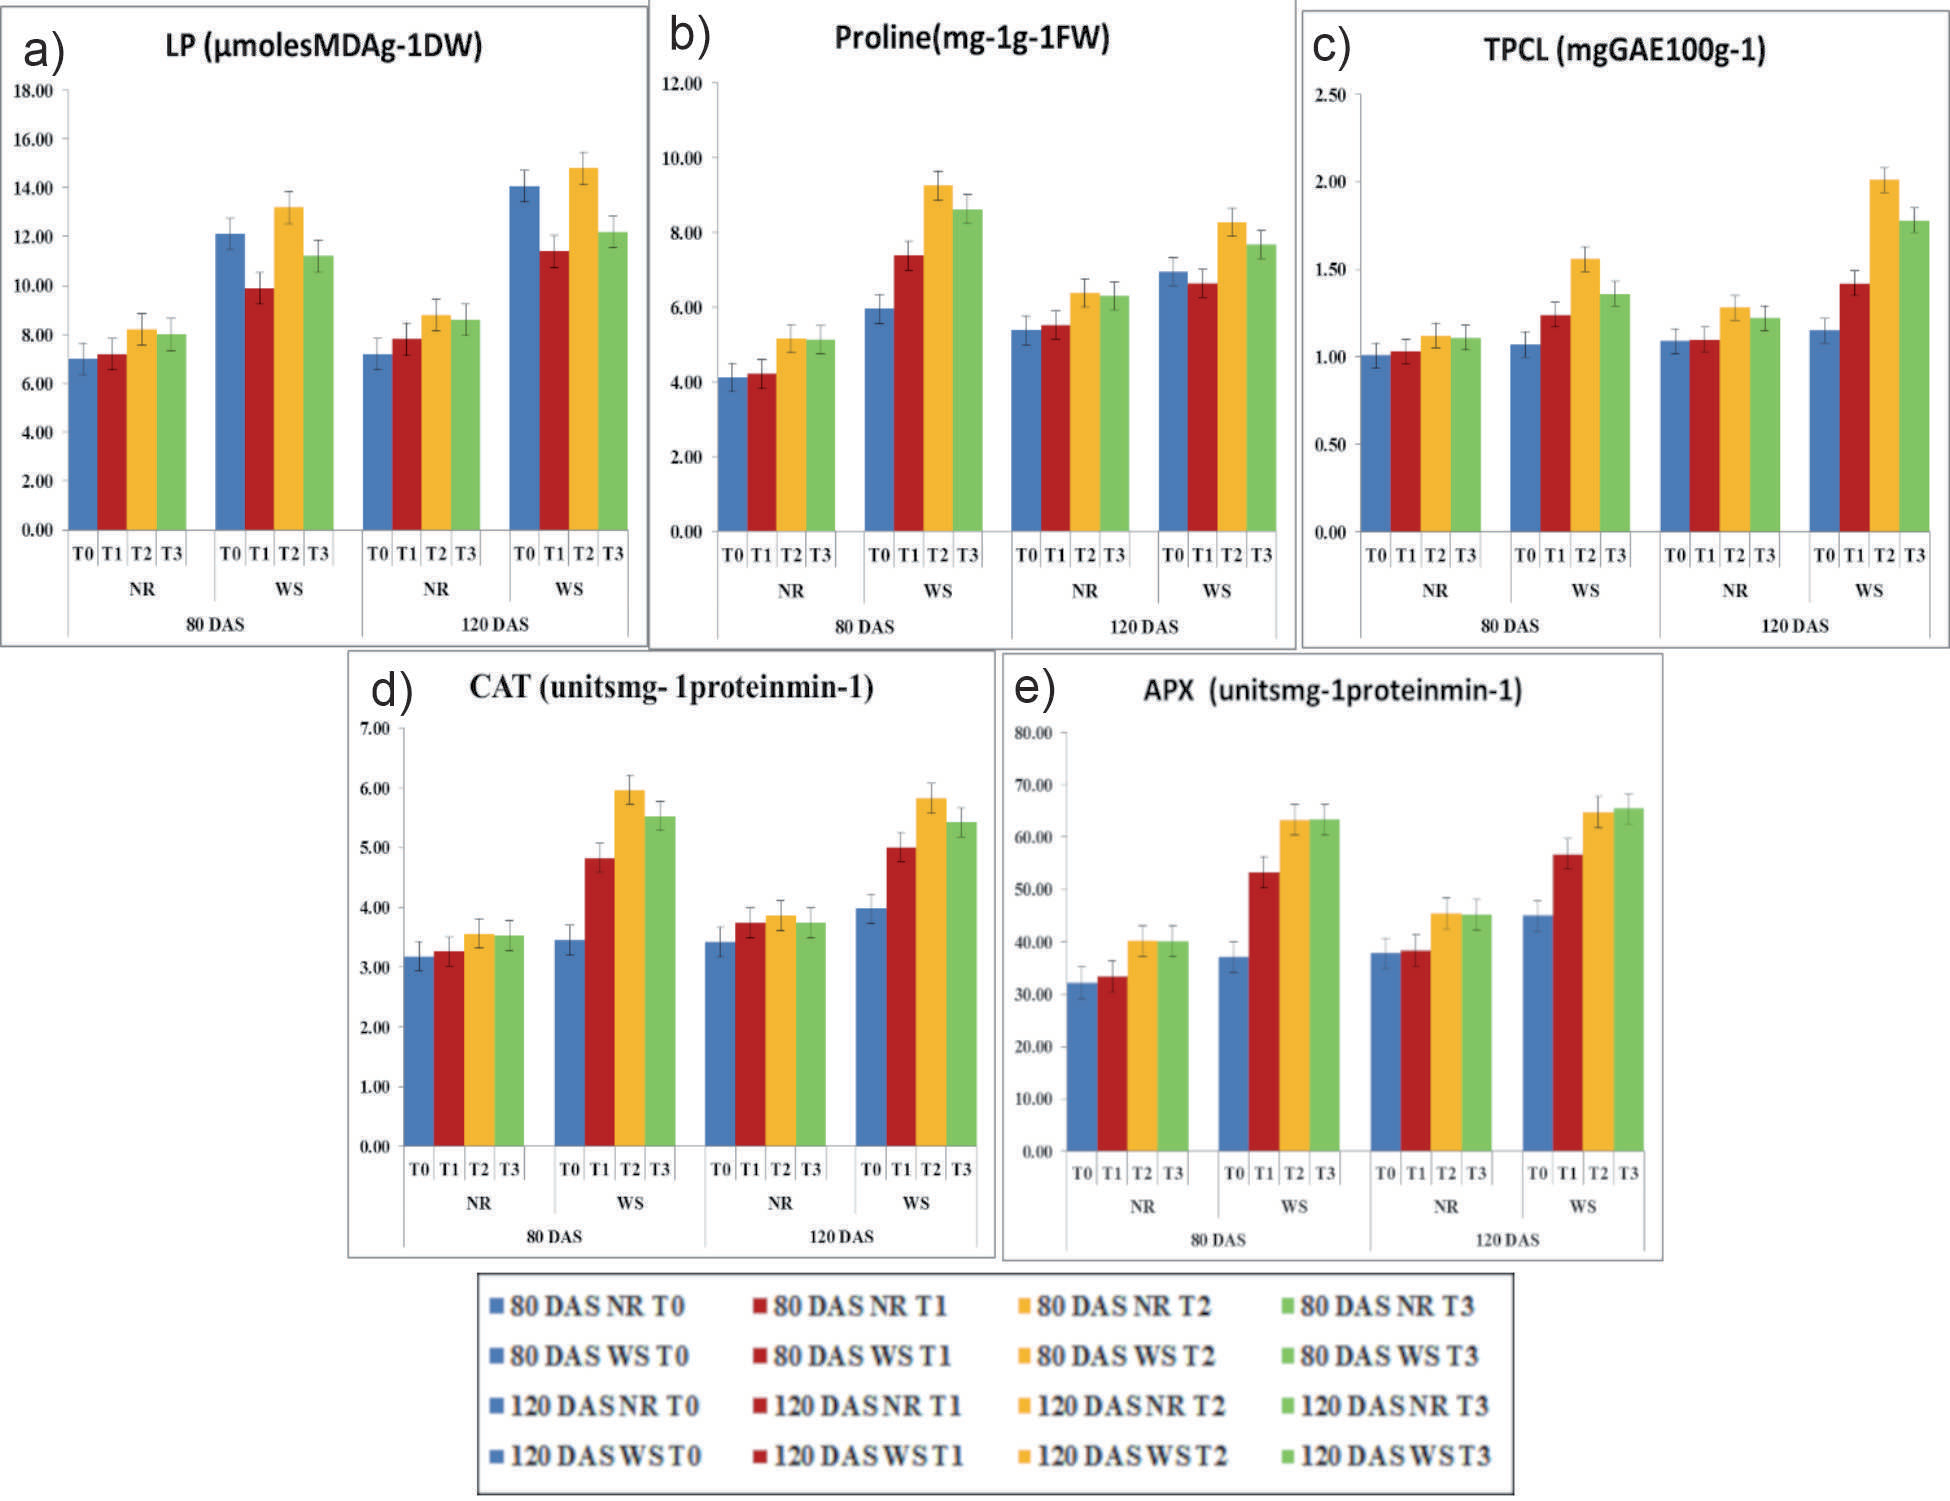
Fig. 5.
Yield and yield-related attributes at varying seed priming treatments at various growth stages under normal vs. water-limiting stress conditions. Data are presented as Mean±S.E. The letters CO: control; NR: normal; WS: water-limiting stress; T0: control/hydroprimed; T1: SA-primed seed; T2: boron-primed seeds; T3: ZnSO4-primed seeds (0.5%); NPP: number of pods plant-1; SI: seed index; EY: economic yield; SY: stover yield; BY: biological yield; HI: harvest index.
Discussion
The present study mainly proposed to explore the seed priming agents’ effect (B, Zn, and SA) on agromorphological and physio-biochemical parameters of chickpea under two priming environments, i.e., irrigated and water-limited stress. The experiment was intended to screen out the most influential priming treatment to mitigate drought stress. The study also focused on exploring the impact of different priming treatments on the overall yield and its related attributes of chickpeas. Being a water and thermosensitive crop, different critical growth stages of chickpea are severely affected due to erratic rainfall/water stress distribution and exceeding temperatures above 35ºC, resulting in hampered yield and production in various areas [46- 48]. The nutritional quality of various legumes, such as lentils [49, 50] and beans, including chickpeas, drastically declined under drought stress, as reported in a few recent studies [51, 52]. The vegetative and pod initiation stages are the most critical for water stress in chickpeas [53]. In comparable paths of erstwhile literatures, our results also confirmed the negative impacts of drought stress at vegetative (pre-anthesis) and reproductive (post-anthesis) stages (40, 80, and 120 DAS), whereas the priming treatments indicated the amelioration effects in aforementioned critical stages under water-limited stress.
Water stress alters the overall morphology and physiology of the plant in terms of agromorphological parameters (growth parameters like plant height, number of branches per plant, number of nodules per plant, and total dry matter accumulation per plant) and physio-biochemical parameters (RWC (%), MSI (%), TCC, TPC, TPCL, APX, and CAT). Reduction in growth parameters is the most primitive and earliest indication of plant-to-water stress [54].
Growth and photosynthesis in plants are positively correlated and ultimately have remarkable effects on yield-associated traits and overall yield under water stress [55-59]. To condense the drastic reduction of yield in chickpeas under water-limited stress, it is vital to evaluate the agromorphological parameters like plant height, number of branches per plant, number of nodules per plant, total dry matter accumulation, and total chlorophyll content. Compared with individual priming treatments, a gradual decrease in the plant’s growth parameters was observed in both chickpea’s pre-anthesis (vegetative) and post-anthesis (reproductive) stages during the stress period. The decline in agronomic parameters in post-anthesis stages under water-stressed conditions is mainly due to the deterioration of pollen grain viability, their germination on the stigma, and pollen tube growth, ultimately resulting in poor flower and pod formation [60, 61].
Fig. 6.
Cluster dendrogram for the estimated traits with varying seed priming treatments, where a) and b) are under normal conditions and c) and d) are under water-limiting stress conditions at 80 and 120 DAS, respectively. The letters CO: control; NR: normal; WS: water-limiting stress; T0: control/hydroprimed; T1: SA-primed seed; T2: boron-primed seeds; T3: ZnSO4-primed seeds (0.5%); PH: plant height; TNNP: total number of nodules plant−1; TNBP: total number of branches plant−1; DWP: dry weight plant−1; RWC: relative water content; MSI: membrane stability index; TCC: total chlorophyll content; LP: lipid peroxidation; TPCL: total phenolic contents; CAT: catalase activity; APX: ascorbate peroxidase activity.
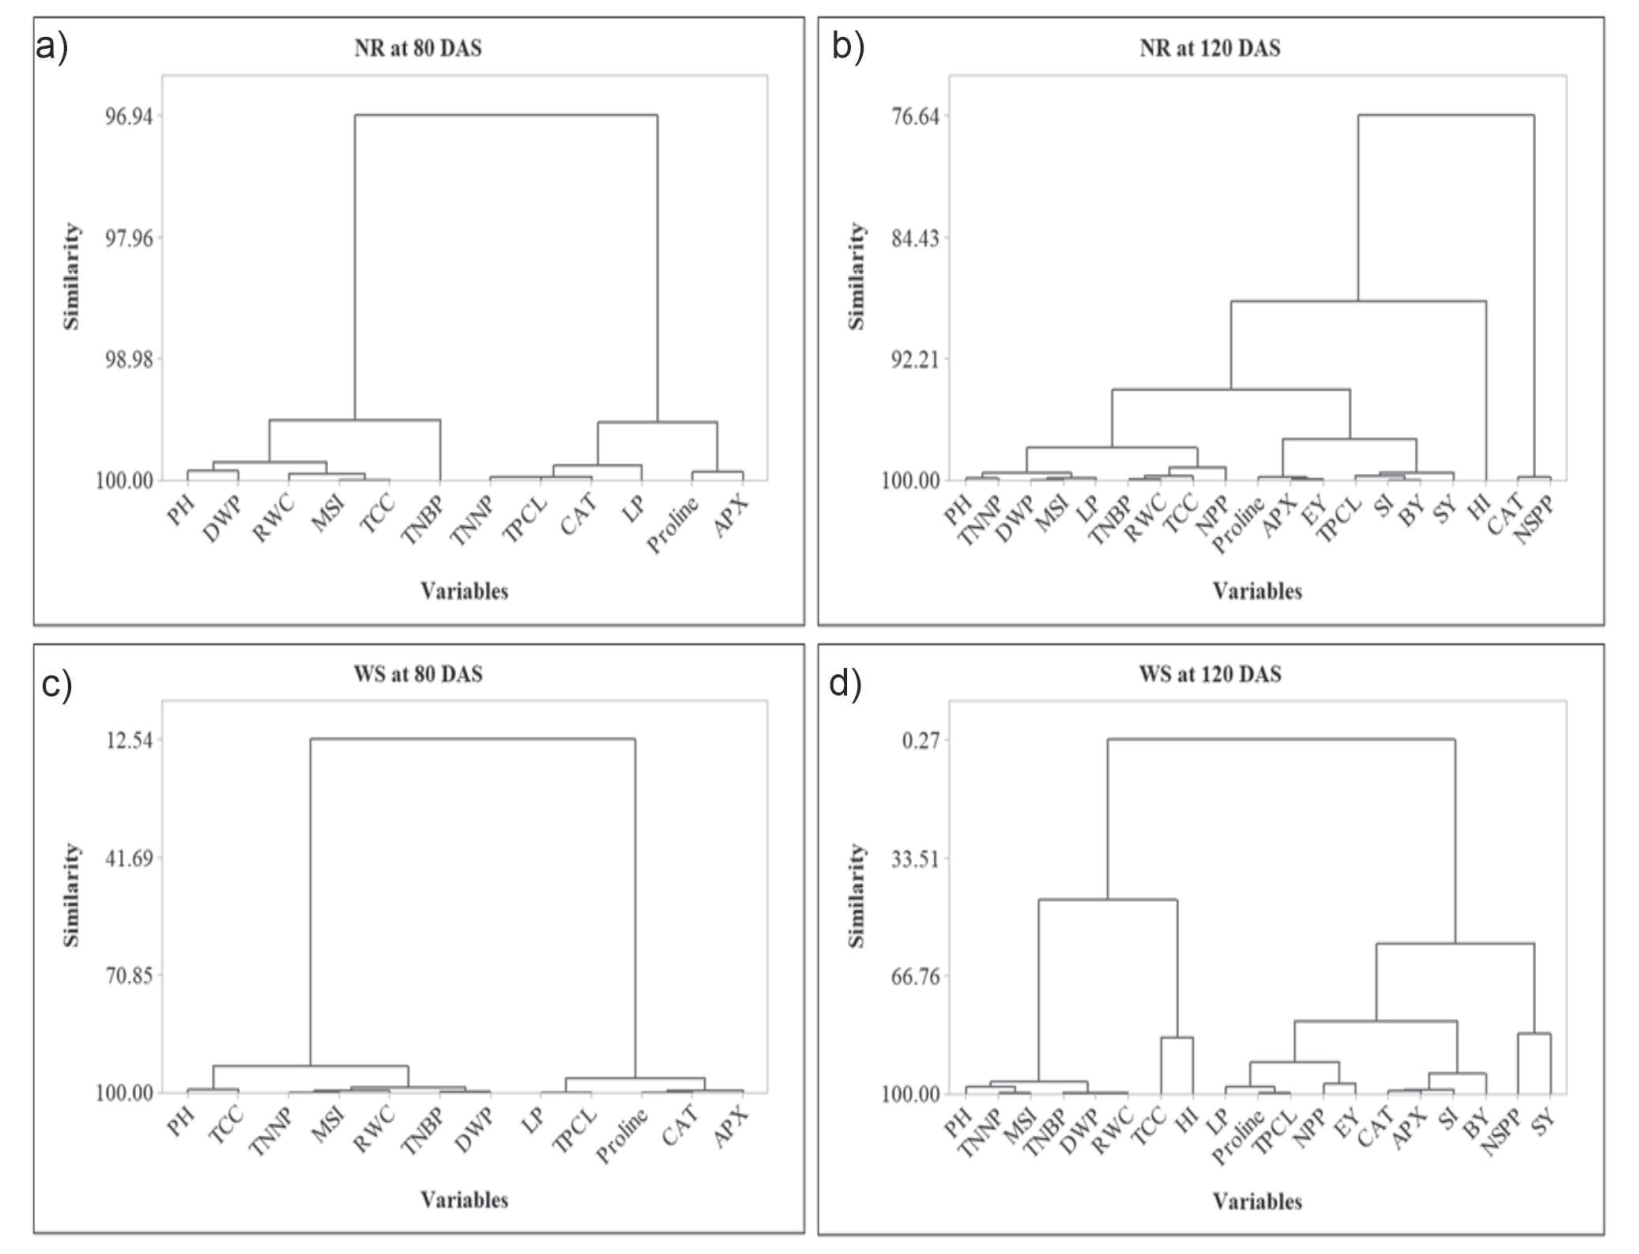
Fig. 7.
Principal component analysis of the estimated traits with varying seed priming treatments, where a) and b) are under normal conditions and c) and d) under water-limiting stress conditions at 80 and 120 DAS, respectively. The letters CO: control; NR: normal; WS: water-limiting stress; T0: control/hydroprimed; T1: SA-primed seed; T2: boron-primed seeds; T3: ZnSO4-primed seeds (0.5%); PH: plant height; TNNP: total number of nodules plant−1; TNBP: total number of branches plant−1; DWP: dry weight plant−1; RWC: relative water content; MSI: membrane stability index; TCC: total chlorophyll content; LP: lipid peroxidation; TPCL: total phenolic contents; CAT: catalase activity; APX: ascorbate peroxidase activity.
A sudden fall in turgor pressure results in a drastic reduction in various agromorphological parameters in various crops under water-stress treatments. This could be due to a reduction in meristematic cell division and expansion in different parts of plants. The disturbance and obstruction in the water flow from the xylem to the adjacent cells lead to a pause in cell elongation [57]. The growth parameters were severely affected when cell elongation, mitosis, and expansion were not in parallel paths.
Reduction in the number of pods, grains per plant, and grain size was positively correlated with reduction in grain yield under water stress conditions [62]. The triggering effect on yield reduction under stressful environments started with the pod initiation stage, which is further manifested by a decrease in the seed filling duration or pace [63]. Cohen et al. [64] highlighted that under drought-stressed environments, the life cycle of pulses may be shortened with premature and reduced numbers of seed production with less vegetative biomass, and this also results in disruption of carbon assimilation and its transport in seeds.
Zn and B application significantly impact chickpeas’ vegetative growth [65], as both micronutrients are essential in the structural integration of cells, cell division, and cell wall synthesis, which could contribute to higher DM production and greater yields. Zn application in soil increased the growth parameters in chickpea [66], and therefore, at the harvesting stage, plots with Zn fertilization had maximum total DW [67], primarily due to a higher number of pods per plant and DW per plant. In addition, Zn fertilization in treatments also increased the DW of roots [68]. Moreover, the priming treatments may be responsible for high intrinsic seed micronutrient reserves [69], which could be supportive in improving seed vigor, germination, stand establishment, and growth parameters under water-limited stress. Our results also revealed significant growth parameter values in micronutrient-priming treatments under individual and stressed conditions compared with the control.
Root nodulation is an important factor in fixing atmospheric nitrogen and absorbing nutrients from the soil in legumes [70]. Water-limited stress might result in altering the morphological structure of rhizobia, ultimately decreasing the infection rate and formation of nodules. Similar results were also pointed out in our study in terms of a decrease in nodulation under water-limited priming treatments. B augments the nitrate levels and has a pivotal role in nitrogen (N) metabolism [71]. It also improves nutrient uptake, root development, and the symbiosis between the plant and nitrogen-fixing bacteria, resulting in increased nodule formation and improving the plant’s capability to absorb and utilize nitrogen. Therefore, incorporating boron seed priming techniques can be a valuable strategy to promote nodulation and nitrogen fixation in chickpea cultivation. Our study revealed the maximum number of nodules in the individual B and Zn priming treatments, whereas a significant number of nodules were also found in the water-stressed priming treatments. The erstwhile literature also underlined the role of B fertilizers in rhizobial N fixation, actinomycetes symbiosis, and cyanophyceae heterocyst formation in leguminous crops [72].
Declining values of total chlorophyll content (TCC) under water-limited stress were due to significant changes in the leaf morphological structures (leaf thickness and leaf size) and anatomical structures (palisade tissue and spongy tissues) [73-75], chlorophyll degradation, and photo-oxidation of chlorophyll pigments [76]. Turgor loss during water stress conditions results in the collapse of mesophyll cell activity and partial stomatal closure [77]. Photo-oxidation and chlorophyll degradation reduced the chloroplastic light-harvesting capacity, ultimately reducing photosynthesis. Therefore, lower values of total chlorophyll content were recorded in water stress priming treatments compared with individual priming treatments. B and Zn showed significant results in total chlorophyll content among stressed treatments. Both micronutrients were necessary for regulating the chlorophyll and carotenoid synthesis, which ultimately protects the photosynthetic machinery [78], increases the activity of carbonic anhydrase by 2-fold [79], and repairs photosystem II [80]. Therefore, the total chlorophyll content values were in line with the aforementioned studies in individual and water stress priming treatments.
RWC and MSI are important and commonly indicative parameters used to evaluate crops against drought tolerance. Water loss from tissues under water deficit can severely affect RWC and MSI [81]. Therefore, both parameters were affected under water stress priming treatments compared with individual priming. However, B and Zn revealed amelioration effects under stressed conditions and showed significant values compared with SA-treated plants. The amelioration impacts could be due to the structural and integral role of B and Zn in cell membranes and cell walls, enhancing the activities of membrane-associated enzymes and reducing lipid peroxidation, hence maintaining the RWC and MSI levels in plants. Boron priming enhances the plant’s water retention capacity by improving water uptake efficiency, reducing transpiration rates, and increasing the water-holding capacity of cells [82-84]. The ability of a plant to conserve and withstand higher RWC for most of the growth stages in the plant life cycle under stress conditions could be an adaptive feature.
The main physiological plant response against drought stress is oxidative damage, which produces increased ROS levels [85]. These ROS are directly responsible for lipid peroxidation in cell membranes [86- 88]. Generally, ROS are present in plants as signaling agents, but upon the advent of stress. Plants prepare themselves against stresses by activating antioxidant defensive machineries (enzymatic and non-enzymatic) to ameliorate the damaging effects of signaling molecules, i.e., ROS [85, 88]. The enzymatic antioxidants that neutralize the levels of ROS include superoxide dismutase (SOD), ascorbate peroxidases (APX), peroxidases (POX), catalase (CAT), and polyphenol oxidases (PPO) [89-91]. However, some non-enzymatic molecules are responsible for osmotic regulation, which includes the accumulation of osmolytes like soluble sugar, proline, soluble protein, etc., in plants under water deficit [92]. The accumulation of proline in cells as an osmotic adjustment agent signals the first reaction to water stress [92, 93] that scavenges the free radicals, modifies cell organelle function, and cushions cellular redox potential [94]. Higher proline content is directly correlated to higher water potential maintenance in leaves, which ultimately keeps antioxidant defense machinery functional. In our results, individual priming treatments revealed lower enzymatic and non-enzymatic antioxidant activity levels than water-stressed plants. However, B and Zn priming treatments under stressed conditions confirmed the higher values of antioxidants (total phenolic content) and antioxidant enzymes (CAT, APX) compared with SA treatment [95-97] and testified that the enhanced activities of antioxidant enzymes (POX, CAT, APX, and osmolytes) against ROS in Ajowan plants under water deficit milieu [97]. CAT and APX enzymes both acted upon the enhanced values of hydrogen peroxide and neutralized its effects in cells by converting H2O2 to H2O and O2.
The priming treatments, especially B and Zn, regulate the total growth parameters of chickpea and prepare the crop plant for the subsequent critical stages (reproductive). B and Zn, as important micronutrients, are pivotal in plant growth, development, and crop nutritional quality [68]. Boron micronutrients play a critical role in the reproductive phases of plants, such as flowering, pollination, fruit setting, seed setting, and grain filling [98]. Moreover, Zn is important in plant reproduction, particularly flower initiation, floral development, male and female gametogenesis, fertilization, and seed development [98]. Zinc deficiency impairs pollen function, fertilization, and ultimately crop yield [99]. Consistent with the above studies, our results confirmed that B and Zn priming treatments helped mitigate the water stress by maintaining the balance between the physiological and morphological parameters in terms of the significant values recorded in the results.
Conclusions
The present study mainly proposed to explore whether the micronutrients (B, Zn) and hormonal priming (SA) are directly involved in the mitigation of water-limited stress through morpho-physiological and biochemical manifestations in the chickpea drought-sensitive variety (GNG-469). The experiment was intended to screen out the most influential priming treatment to mitigate drought stress. Seed priming was found to be a novel and promising attempt to regulate the antioxidant defense machinery in mitigating the abiotic stress by reducing the levels of ROS formation in cells. The present research also suggests that the increase in lipid peroxidation in stress-induced plants signals for cell membrane leakage, which further correlates with a reduction in drought-stressed plant yields for chickpeas. Results from the current study provide a better insight that micronutrients B followed by Zn primed seeds significantly improve the growth parameters in terms of plant height, total dry weight plant−1 (DWP), total number of branches plant−1 (TNBP), total number of nodules plant−1 (TNNP), biochemical parameters (free proline content and total phenolic content), physiological parameters (total chlorophyll content, relative water content, and membrane stability index), and yield characteristics (number of pods plant-1, seed index, economic yield, stover yield, biological yield, and harvest index) under water-stressed environments. Furthermore, the SA priming treatment showed less protection than boron and Zn-primed seeds. The present study clearly indicated that the role of nutria-priming is more promising in ameliorating abiotic stress in chickpeas than hormonal priming. Furthermore, the utilization and better understanding of different priming chemicals with varying durations in molecular mechanisms were also an effective approach and provide additional opportunities to exhibit effective agronomical improvements for sustainable food production.

