

Introduction
Recently, the human population has increased and human activities have intensified, exacerbating eutrophication in lakes, which has become a topic of increasing concern [1]. Eutrophication triggers algal blooms and simplifies the food web, which reduces biodiversity and causes substantial harm to the aquatic ecosystem [2]. Hence, addressing the eutrophication of water bodies is now crucial for mitigating water pollution. Currently used methods for managing water eutrophication involve physical, chemical, and biological remediation technologies [3]. However, despite the high costs involved, physical remediation often fails to eradicate the root cause effectively [4]. Further, chemical remediation yields rapid results but also leads to secondary pollution of the aquatic environment [5]. Using bioremediation technology for the restoration of lakes, including artificial wetlands and aquatic plant restoration, has attracted increasing attention, as it causes minimal secondary pollution, thereby reducing the harmful impact on the environment [6, 7]. However, these technologies lead to slow plant growth and prolonged repair cycles.
Submerged macrophytes play an important role in water purification as they contribute to the restoration of the water ecosystem and maintain its health by reducing the levels of pollutants, including nitrogen, phosphorus, and organic matter, through enrichment, adsorption, and oxidation decomposition [8, 9]. The type and characteristics of substrates in a lake markedly influence the restoration and reconstruction of its ecosystem, providing the fundamental conditions for submerged plant growth and development as well as stable colonization [10]. Reportedly, eutrophic sediments inhibit the growth of submerged macrophytes [11]. Therefore, selecting environmentally friendly and economically viable materials to improve the conditions at the bottom of the lake is crucial for promoting submerged macrophyte growth and restoring lake ecosystems.
Maifanite, a natural silicate mineral, is known to gradually release essential mineral elements, such as potassium ions, calcium ions, and magnesium ions (Mg2+), when immersed in water, albeit often in low concentrations [12]. These mineral elements play a pivotal role in the growth, development, and reproduction of plants and microorganisms [13]. Magnesium is an essential element for carbohydrate allocation, and its deficiency can alter the expression of the gene encoding magnesium transporter, resulting in delayed plant growth and changes in biomass allocation between roots and stems [14]. Therefore, an appropriate increase in Mg2+ concentration can positively affect plant growth and root development [15] and significantly improve plant root biomass as well as nitrogen and phosphorus absorption [16].
A previous study reported that the presence of substrates can reduce the nutrient load within the sediment and aid in controlling the resuspension of sediments at the bottom of the lake [17]. However, there are only a few reports on the effects of mineral element-loaded modifications of substrates on plants. Therefore, it is necessary to investigate the direct and indirect impacts of mineral-loaded substrates on submerged plants and rhizosphere microorganisms. The outcomes of this investigation can be used to guide the application of substrate modification for the restoration of water bodies.
In this study, maifanite loaded with Mg2+ was used as a substrate to improve the quality of lake sediments. Different doses of modified maifanite were added to the sediment and the effect on submerged macrophytes was observed. The study objectives were (1) to explore the influence of mineral elements on the growth and physiological indicators of submerged macrophytes and (2) to compare the effects of different doses of modified maifanite on microorganisms in the rhizosphere environment of submerged macrophytes.
Materials and Methods
Study Site and Sediment Collection
Jinyin Lake (114º07′N, 30º38′E) is a typical eutrophic shallow lake with an average depth of 2.5 m and a surface area of 0.77 km2. This lake is situated in the middle reaches of the Yangtze River in Wuhan, Hubei Province, China. In May 2023, the pH, dissolved oxygen (DO), and water temperature of the overlying water in shallow (1 m deep) areas were measured using a YSI EXO2 Multi-Parameter Water Quality Analyzer (YSI Inc., Yellow Springs, OH). Further, overlying water and surface sediment samples from 10 cm below the surface were collected using a Peterson sampler, stored in sterile zip-lock bags, and transported to the laboratory on ice. The samples were then stored at 4°C before further physical and chemical analyses as described by Wang et al. [18]. The pH, DO, total phosphorus (TP) content, total nitrogen (TN) content, and chemical oxygen demand of the overlying water were 9.58, 10.29 mg L-1, 0.15 mg L-1, 0.81 mg L-1, and 25.32 mg L-1, respectively, whereas organic matter, TP, and TN contents in the dry sediment were 56.8 g kg-1, 1.79 g kg–1, and 2.87 g kg-1, respectively.
Materials
Washed maifanite (particle size: 3–5 mm) was modified by mixing it with a 1.5 mol L-1 MgCl2 solution, followed by the addition of a 25% NaOH solution to adjust the pH of the mixture to 11. The maifanite was soaked for 5 h, dried at 110°C for 10 h, washed with distilled water until the pH of the washing water reached 7, and finally dried at 60°C to obtain the modified maifanite. Magnesium chloride hexahydrate (MgCl2·6H2O, 99.8% purity) and sodium hydroxide (NaOH, 96% purity) were obtained from Sinopharm Chemical Reagent Co., Ltd (Shanghai, China). Maifanite was procured from Henan Zhisheng Environmental Protection Technology Co., Ltd (Henan, China).
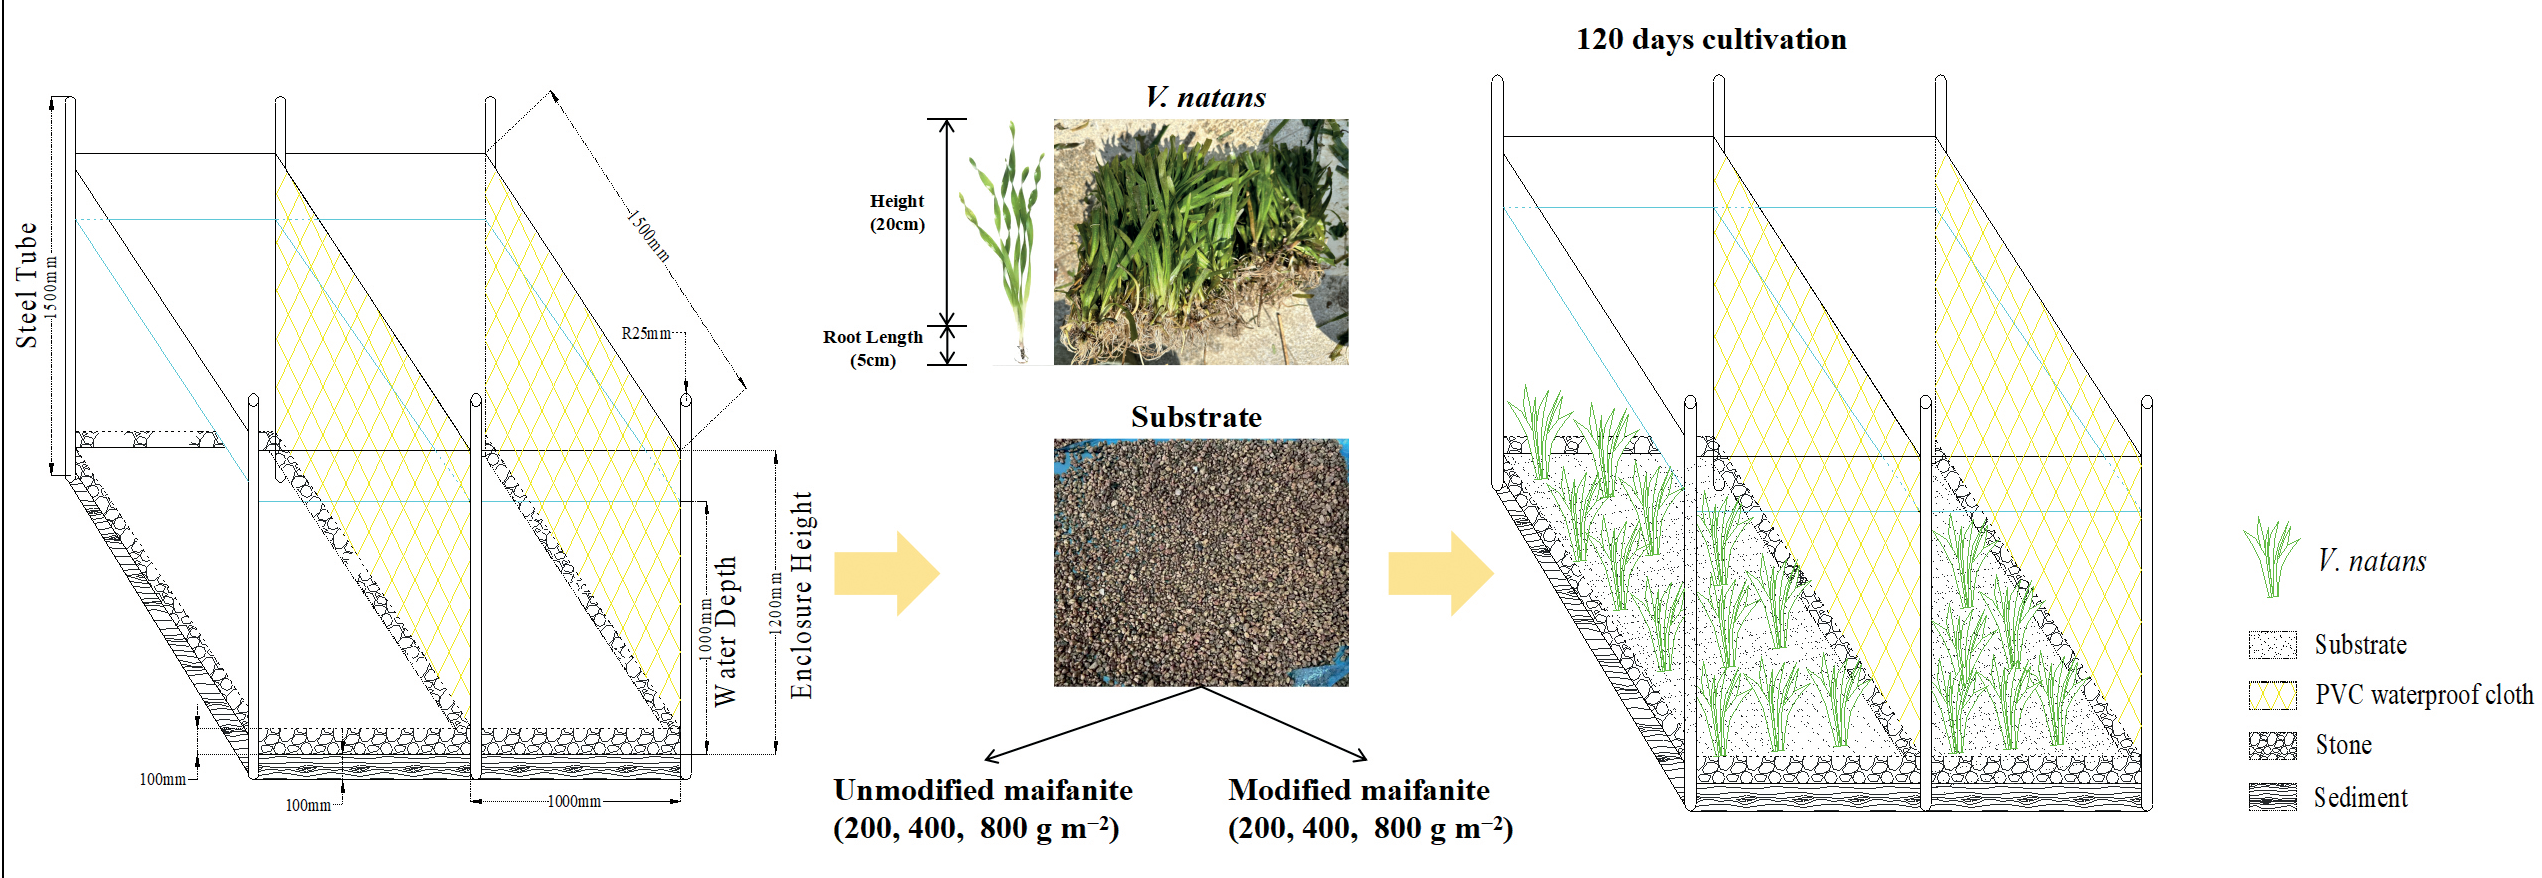
Vallisneria natans (Lour.) Hara, a dominant aquatic plant growing in the middle reaches of the Yangtze River, was selected as the test plant because of its well-developed roots, rapid growth, and ease of cultivation. V. natans plants were initially cultivated for 1 week at 25°C, with a light intensity of 3500 lx and a light-to-shade ratio of 12:12 hours. Subsequently, healthy plants with similar growth conditions were selected, and their roots were trimmed to approximately 5 cm in length. Before planting, the leaves were trimmed to a length of 20 cm, leaving 4–5 leaves; the plants were then transplanted into an enclosure.
Experimental Design and Method
A waterproof PVC enclosure (21.0 m × 1.5 m) was constructed in the sediment collection area. Internally, the enclosure was partitioned into 21 smaller enclosures using PVC plates, each measuring 1.0 m × 1.5 m, and secured at the corners using steel pipes measuring 0.5 m in diameter and 1.5 m in length. The bottom of each enclosure was compacted with a nylon mesh with stones to limit water exchange between the interior and exterior of the enclosure (Fig. 1). Within each enclosure, varying substrate doses were added and V. natans were planted at a density of 60 plants m-2. Groups were labeled based on the amounts of unmodified maifanite added (groups ME1, ME2, and ME3 had 200, 400, and 800 g m-2 of maifanite, respectively). Similarly, 200, 400, and 800 g m-2 of modified maifanite were added to groups MM1, MM2, and MM3, respectively. No maifanite was added to the control (CK) group. Three parallel enclosures were established for each treatment group.
Sampling was performed monthly, with three plants collected randomly from each enclosure. After cleaning the collected samples, their growth and physiological indices were measured. Growth indices included leaf number, plant height, biomass, and new root length, and physiological and biochemical indices included leaf superoxide dismutase (SOD) activity, catalase (CAT) activity, chlorophyll content, malondialdehyde (MDA) content, and root vitality. Leaf SOD and CAT activities were measured using the guaiacol method. Chlorophyll and MDA contents were determined using the Lichtenthaler–Arnon and thiobarbituric acid methods, respectively. Root vitality was evaluated using the triphenyltetrazolium chloride method [19].
Microcosm Experiments
At the end of the experiment, the sediment samples in the enclosure were collected and stored at -80°C for DNA extraction. Genomic DNA was extracted using the Fast DNA Spin Kit for Soil (Qbiogene Inc., USA) following the manufacturer’s protocol. Extracted DNA samples were stored at -20°C after assessing purity and concentration using an ultraspectrophotometer (NanoPhotometer-N60, IMPLEN, Germany). The V3–V4 region of the 16S rRNA gene of the samples was amplified using PCR using primers 341 F (5′-CCTACGGGNGGCWGCAG-3′) and 805 R (5′-GACTACHVGGGTATCTAATCC-3′) [20]. The PCR system (20 μL) comprised 4 μL of 5× FastPfu Buffer, 2 μL of dNTPs (2.5 mmol L-1), 0.8 μL of each primer (5 μmol L-1), 0.4 μL of FastPfu Polymerase, 0.2 μL of BSA, 1 μL of template DNA, and 10.8 μL of ddH2O. The PCR involved initial denaturation at 95°C for 3 minutes, followed by 30 cycles of denaturation at 95°C for 30 s, annealing at 53°C for 30 s, and extension at 72°C for 45 s. The PCR amplification products were purified and quantified using the AxyPrep DNA Gel Recovery Kit (AXYGEN, USA) and QuantiFluoruantTM-ST blue fluorescence quantification system, respectively. Homogenized sequencing libraries were then prepared and subjected to quality inspection. The qualifying libraries were subjected to high-throughput sequencing using a HiSeq 2500 PE250 system.
Statistical Analyses
The physiological and biochemical characteristics of the V. natans samples from different treatment groups were analyzed through one-way ANOVA and Tukey’s test using SPSS 20.0 software. Detrended correspondence analysis revealed gradient lengths of the physiological traits of V. natans shorter than 3.0. Consequently, redundancy analysis (RDA) was performed to examine the relationship between the differences in physiological and biochemical characteristics of V. natans samples across different treatment groups using CANOCO 4.5 software.
Results
Effects of Different Substrates on the Growth Indices of V. natans
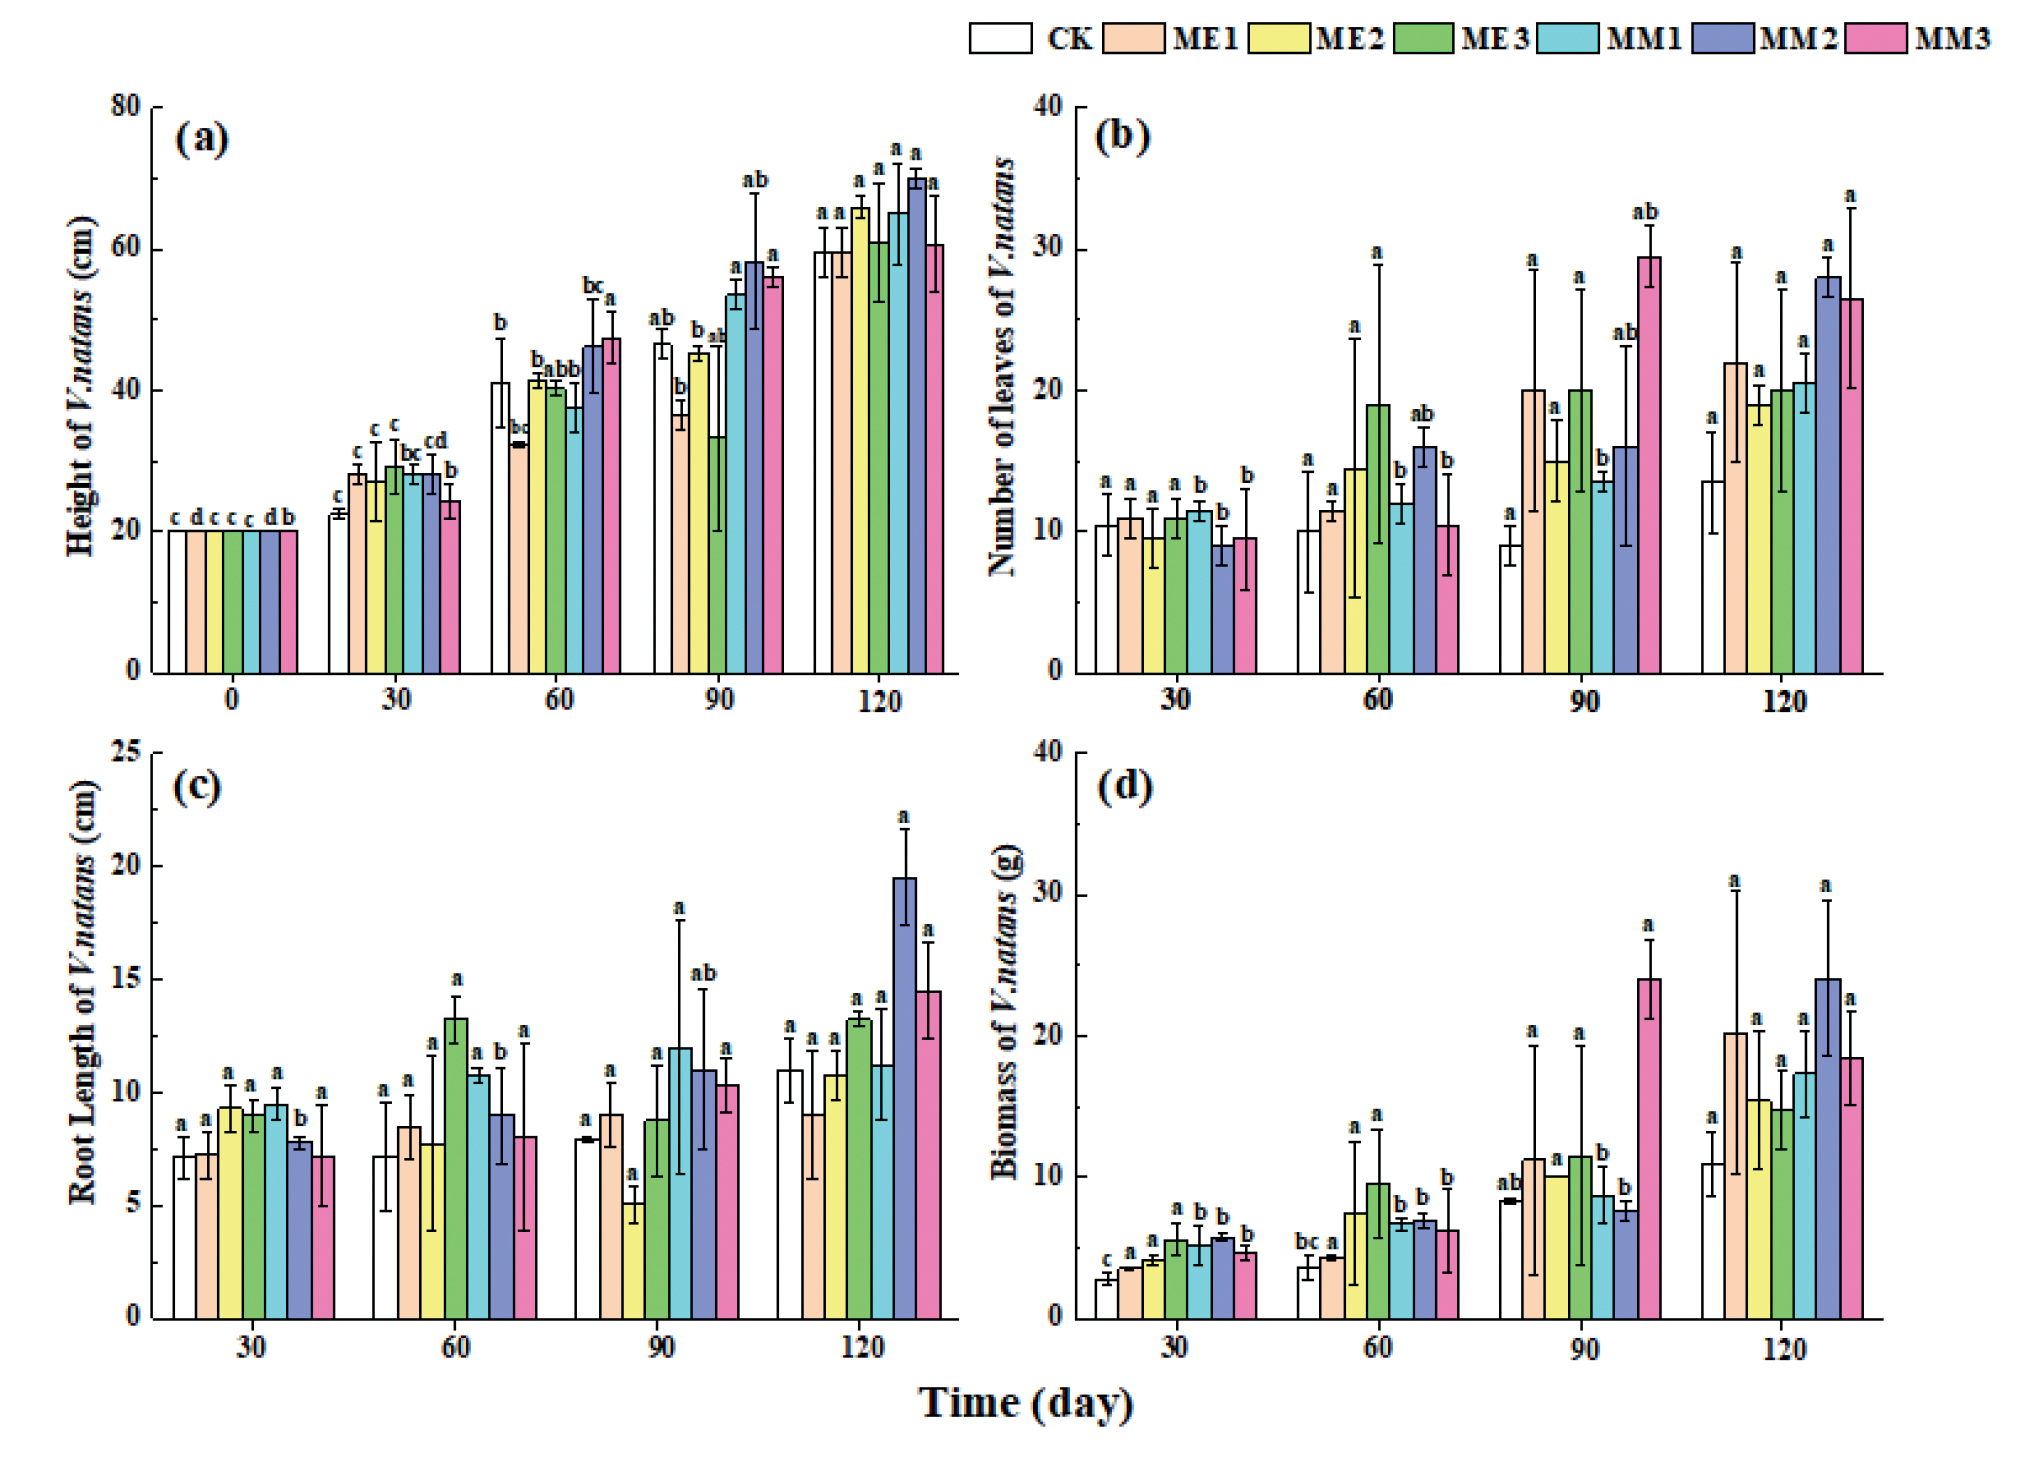
The growth indices of V. natans serve as visual indicators of its growth and development. As depicted in Fig. 2a, the increase in plant height within the same treatment group varied significantly over different time points (P < 0.05). Except in the ME3 group, the increase in plant height in all other groups was positively correlated with culture time. Throughout the culture period, the MM2 group exhibited the maximum increase in height, reaching 50 cm. After 120 days, the number of leaves in the groups with other substrates exceeded that in the CK group (Fig. 2b). Throughout the culture period, the number of leaves in the modified maifanite groups differed significantly (P < 0.05), with the MM3 group exhibiting the highest mean number of leaves.
The root length of the plants in the modified maifanite groups increased compared with that of those in the CK group at each time point, with the MM2 group exhibiting a significant difference (P < 0.05; Fig. 2c) and achieving a maximum root length of 19.5 cm at 120 days. Biomass and leaf number displayed similar trends at 120 days. Specifically, upon the addition of substrate to the submerged macrophyte surface, the biomass of the substrate groups exceeded that of the CK group, and variations in biomass within the same modified substrate treatment group at different times showed significant differences (P < 0.05; Fig. 2d).
Effects of Different Substrates on the Ecophysiological Indices of V. natans
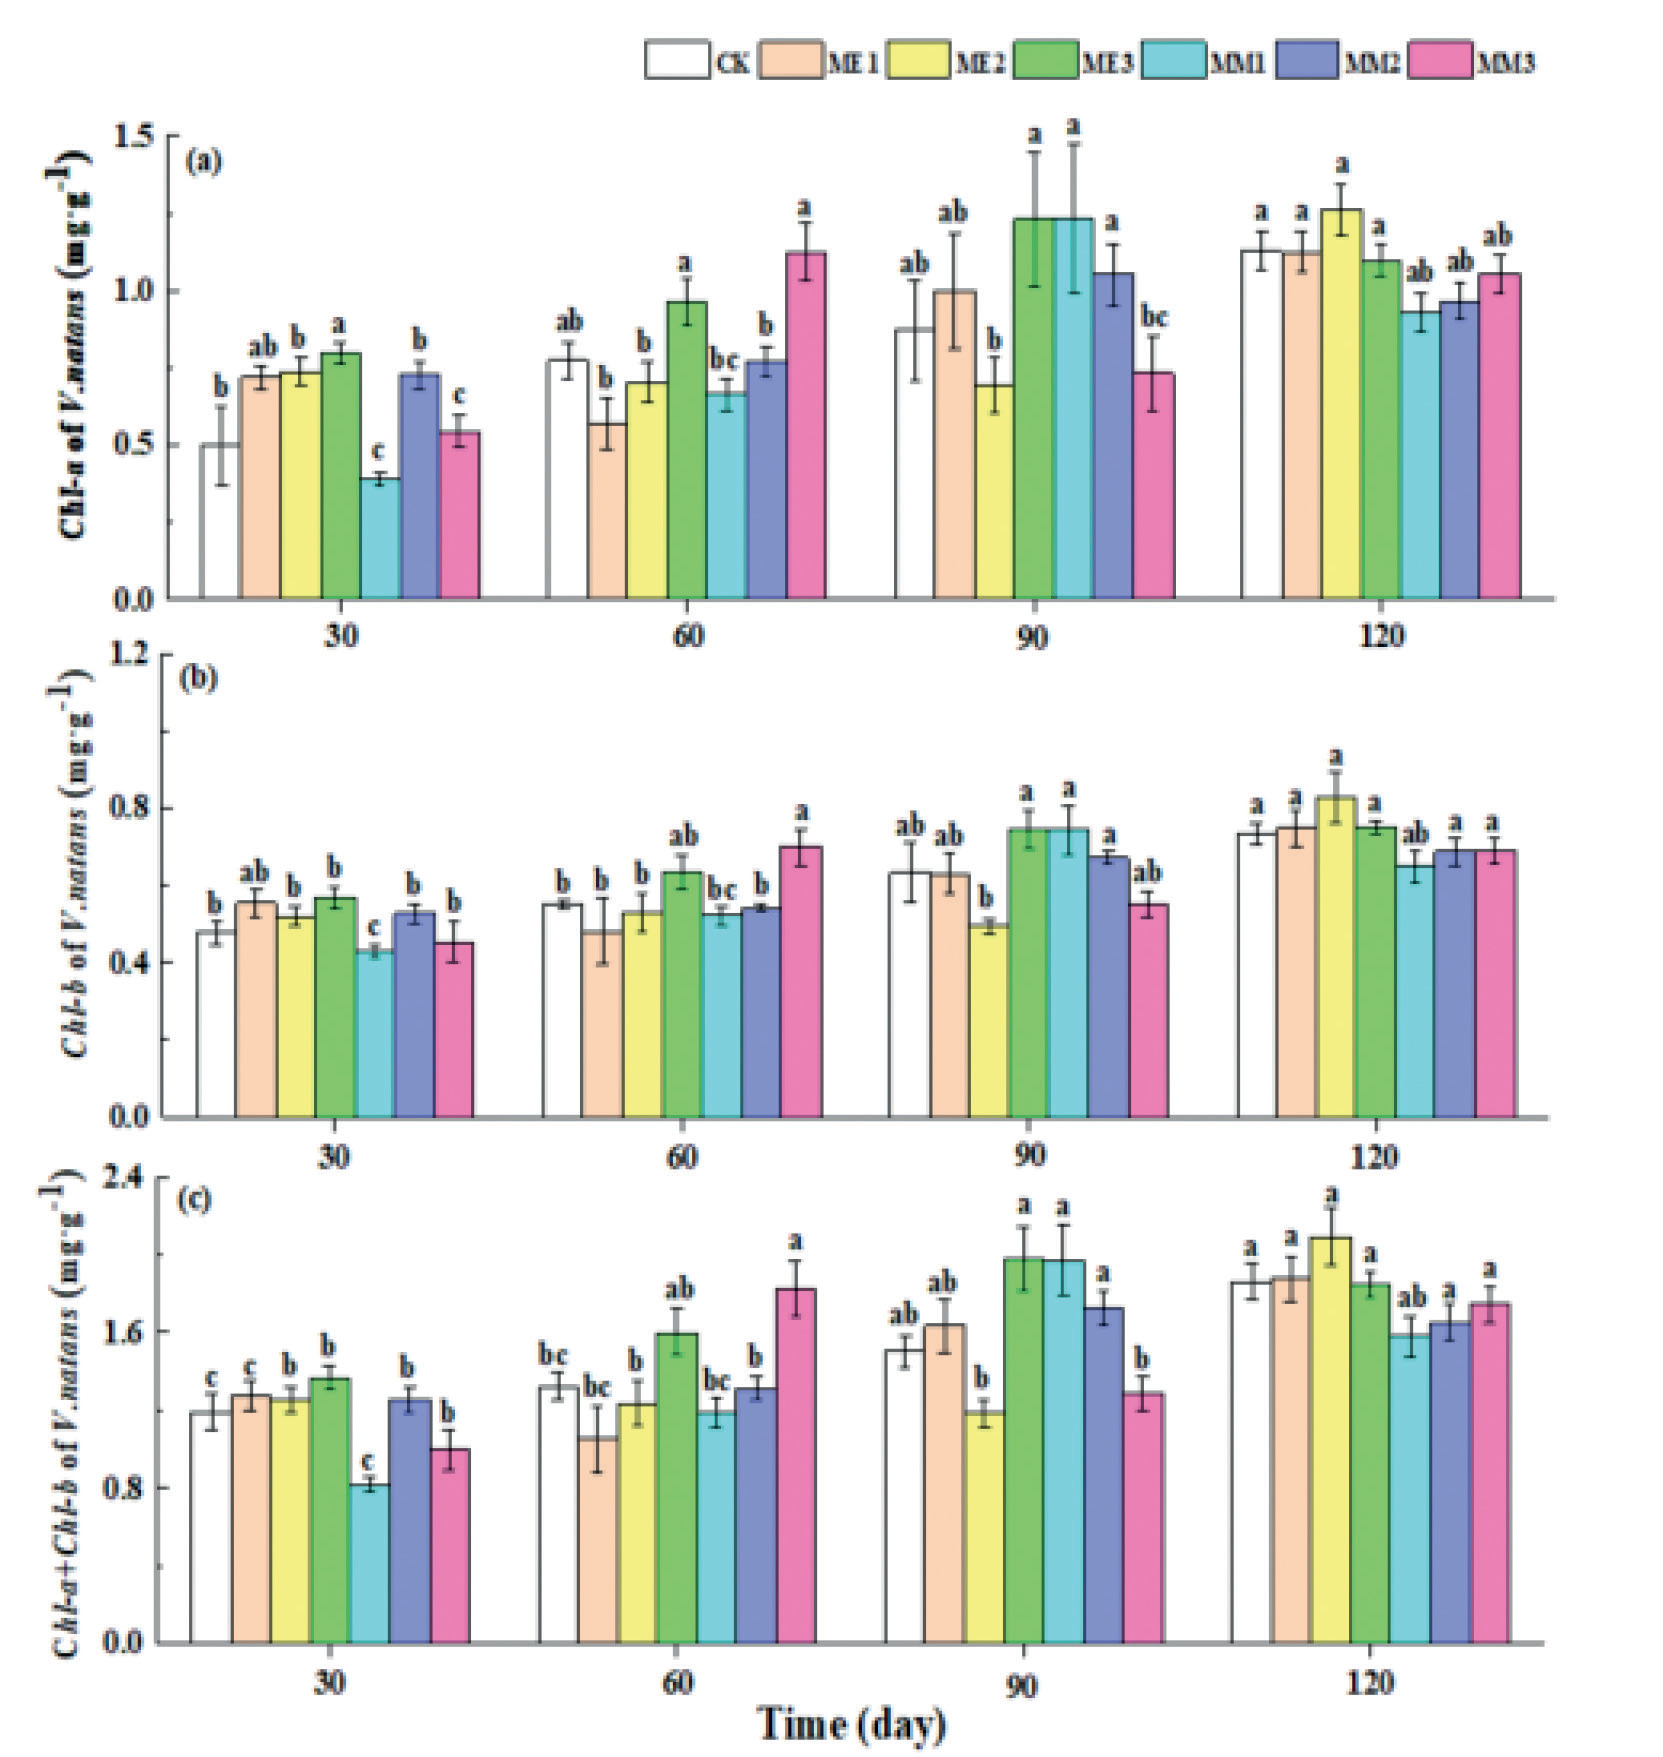
Chl-a content in the leaves of the ME3, MM1, and MM2 groups initially increased, followed by a subsequent decrease with culture time. In contrast, a gradual increase was observed in the CK group (Fig. 3a). Except for the ME3 group, Chl-a content in the same treatment group was significantly different at different culture times (P < 0.05). Similarly, Chl-b content within each treatment group also significantly varied with the duration (P < 0.05). By 120 days, the Chl-b content in the ME2 group reached a maximum at 0.83 mg g-1 (Fig. 3b). The total chlorophyll content across different groups significantly changed with the duration (P < 0.05; Fig. 3c). In the later stages of the culture period (90–120 days), the total chlorophyll content in most groups reached its peak except in the MM3 group.
Fig. 3.
Effects of different maifanite substrates on chlorophyll content in V. natans leaves. Different lowercase letters in the bar chart indicate significant differences at the P < 0.05 (Tukey’s test) level in the same treatment group at different times. Error bars indicate the standard deviation.
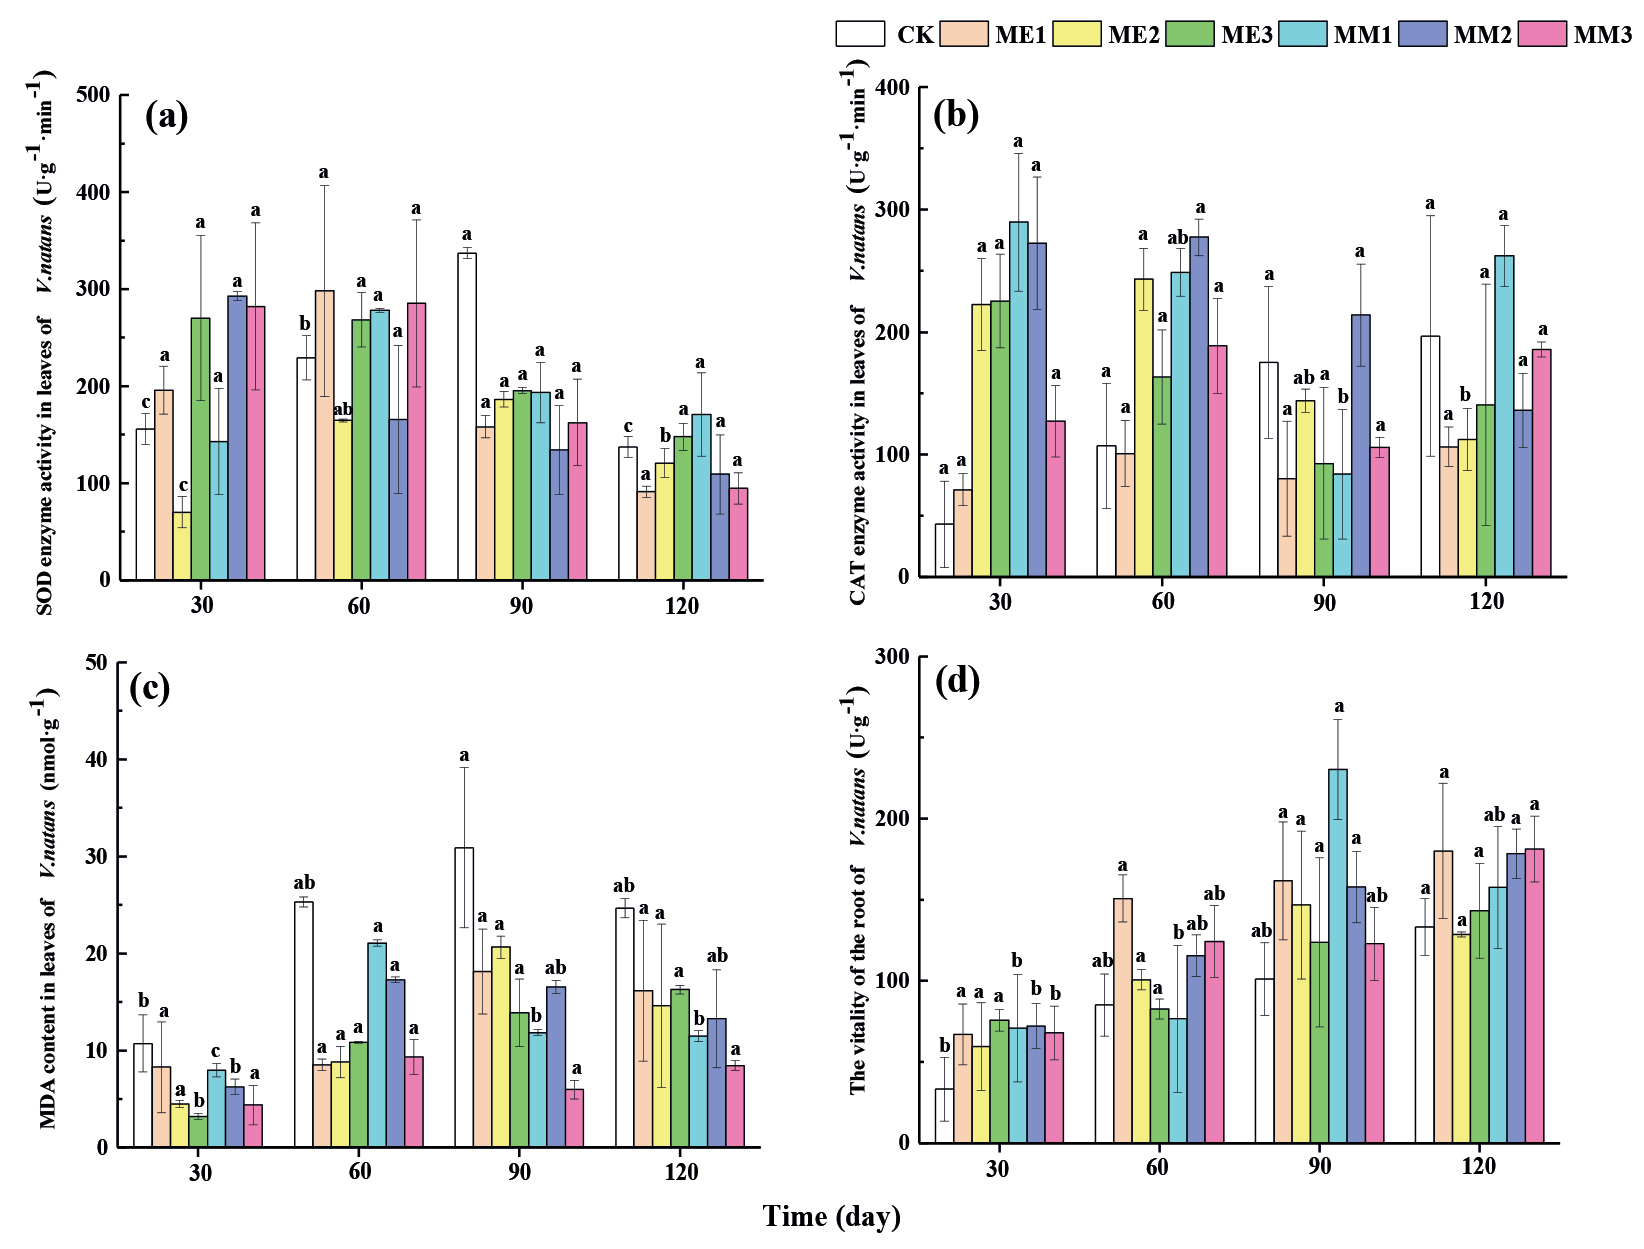
Throughout the culture period, the maximum mean SOD activity in V. natans leaves was 220.42 U g-1 min-1 in the ME3 group (Fig. 4a). The SOD activity in the ME3 and MM2 groups exhibited a similar gradually decreasing trend, whereas that in other groups exhibited an initial increase followed by a decrease. By day 30, the CAT activity in all treatment groups exceeded that in the CK group (Fig. 4b). Over the entire culture period, the mean CAT activities in the modified substrate groups exceeded that in the CK group, with the MM2 group reaching the highest value at 224.9 U g-1 min-1.
Except for the ME3 and MM3 groups, the MDA content in the V. natans leaves initially increased and then decreased. The MDA content in the CK group was significantly higher than that in the treatment groups at each time point (P < 0.05; Fig. 4c). The root vitality of the CK group was consistently lower than that of the ME1, MM2, and MM3 group throughout the experimental period. Root vitalities of the modified substrate groups exhibited significant differences (P < 0.05). In the later stages (90–120 days), root vitalities in the modified substrate groups exceeded that in the CK group (Fig. 4d).
Redundancy Analysis
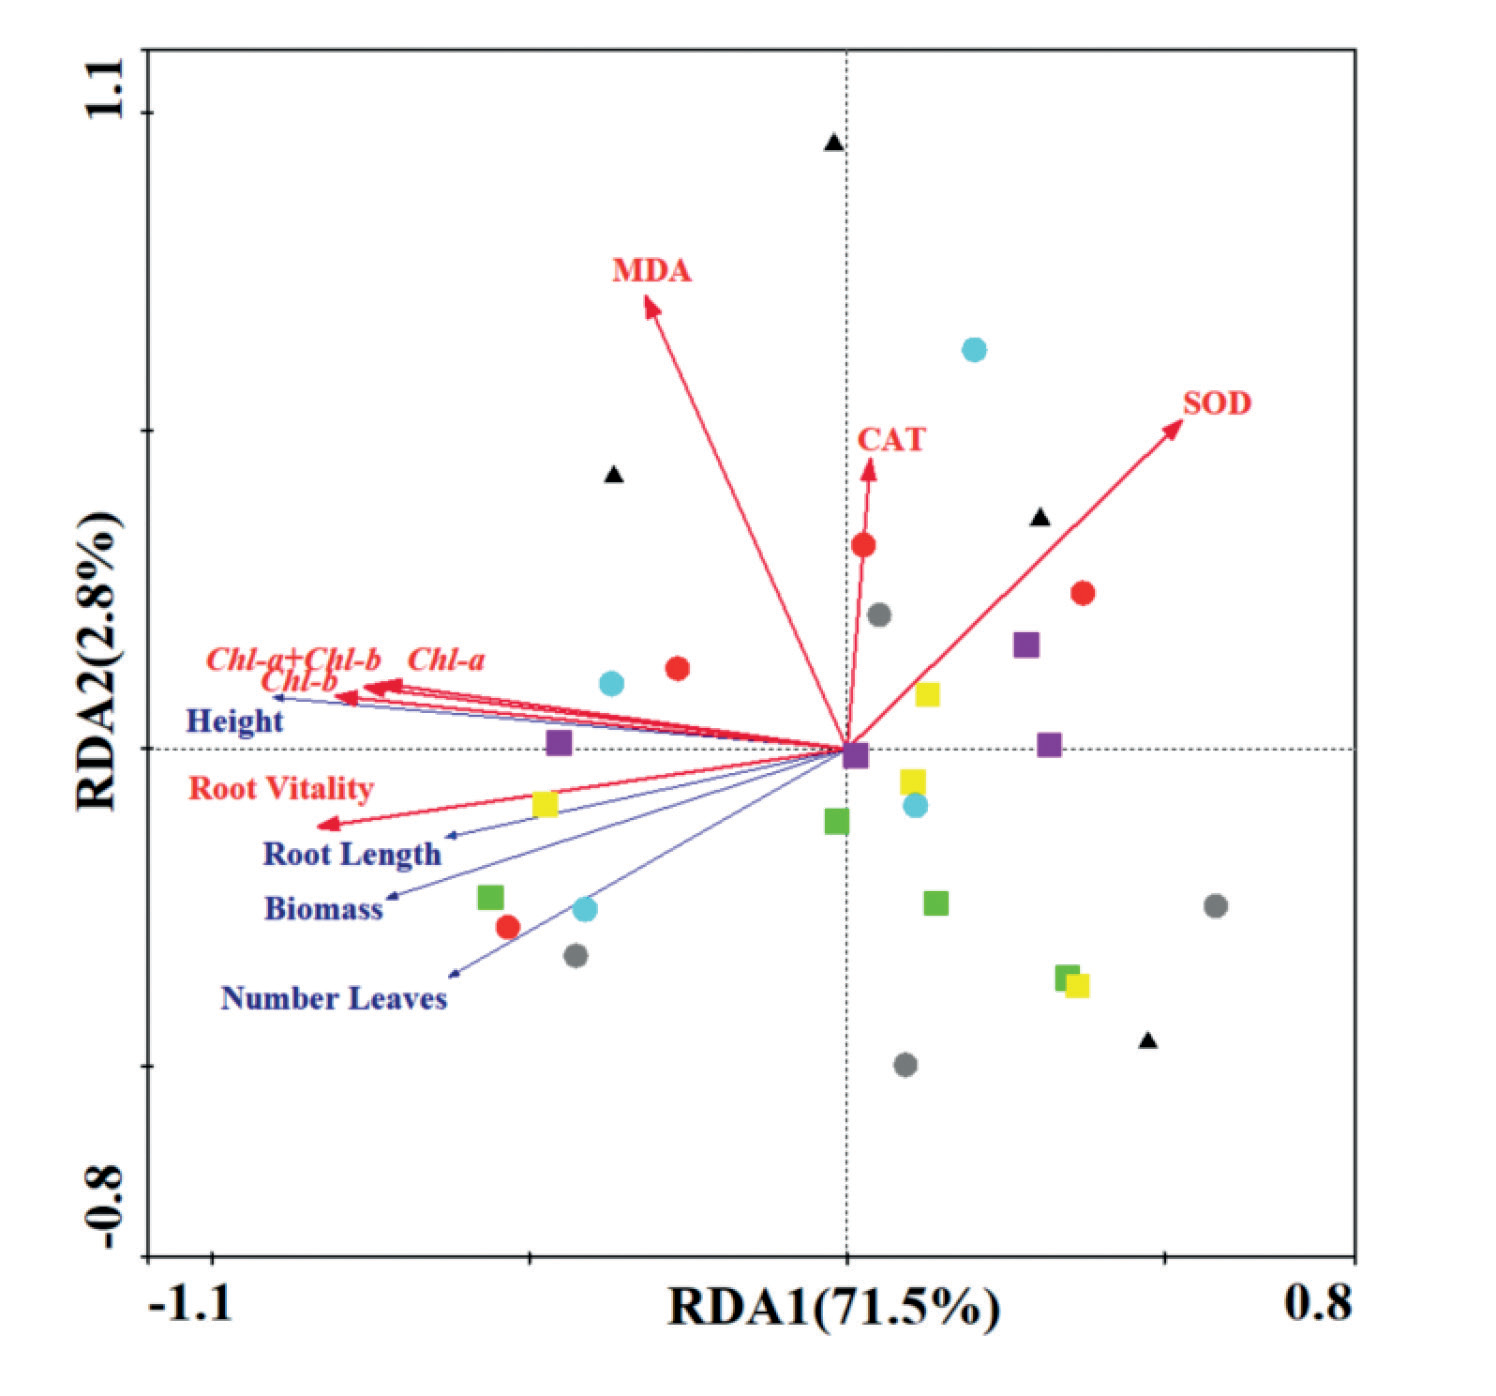
As depicted in the RDA plot in Fig. 5, the first two RDA axes collectively explain 74.3% of the variance. The primary effects of the substrate on the traits of V. natans were in terms of plant height, root vitality, and biomass. Positive correlations were observed between root vitality; Chl-a, Chl-b, and Chl-a + Chl-b content; and growth indicators in all groups, suggesting that substrate improvement can enhance the photosynthetic efficiency of plants. Compared with the unmodified maifanite groups, the modified maifanite groups exhibited closer alignment with the growth and physiological indices of V. natans, indicating that modified maifanite significantly impacts the growth of V. natans. Notably, the MM2 group demonstrated the most pronounced promoting effect on the growth of V. natans.
Effects of Different Substrates on the Rhizosphere Microbial Communities in Sediments
Table S1 presents the influence of substrates on the α-diversity index of the microbial community. Following substrate addition, the Simpson index varied across all groups, although with minimal changes compared with the CK group. The Shannon index for all substrate groups exceeded that of the CK group. The Chao, ACE, and Sobs indices of the modified maifanite groups exceeded those of the unmodified maifanite and CK groups, with the MM2 group exhibiting the highest values.
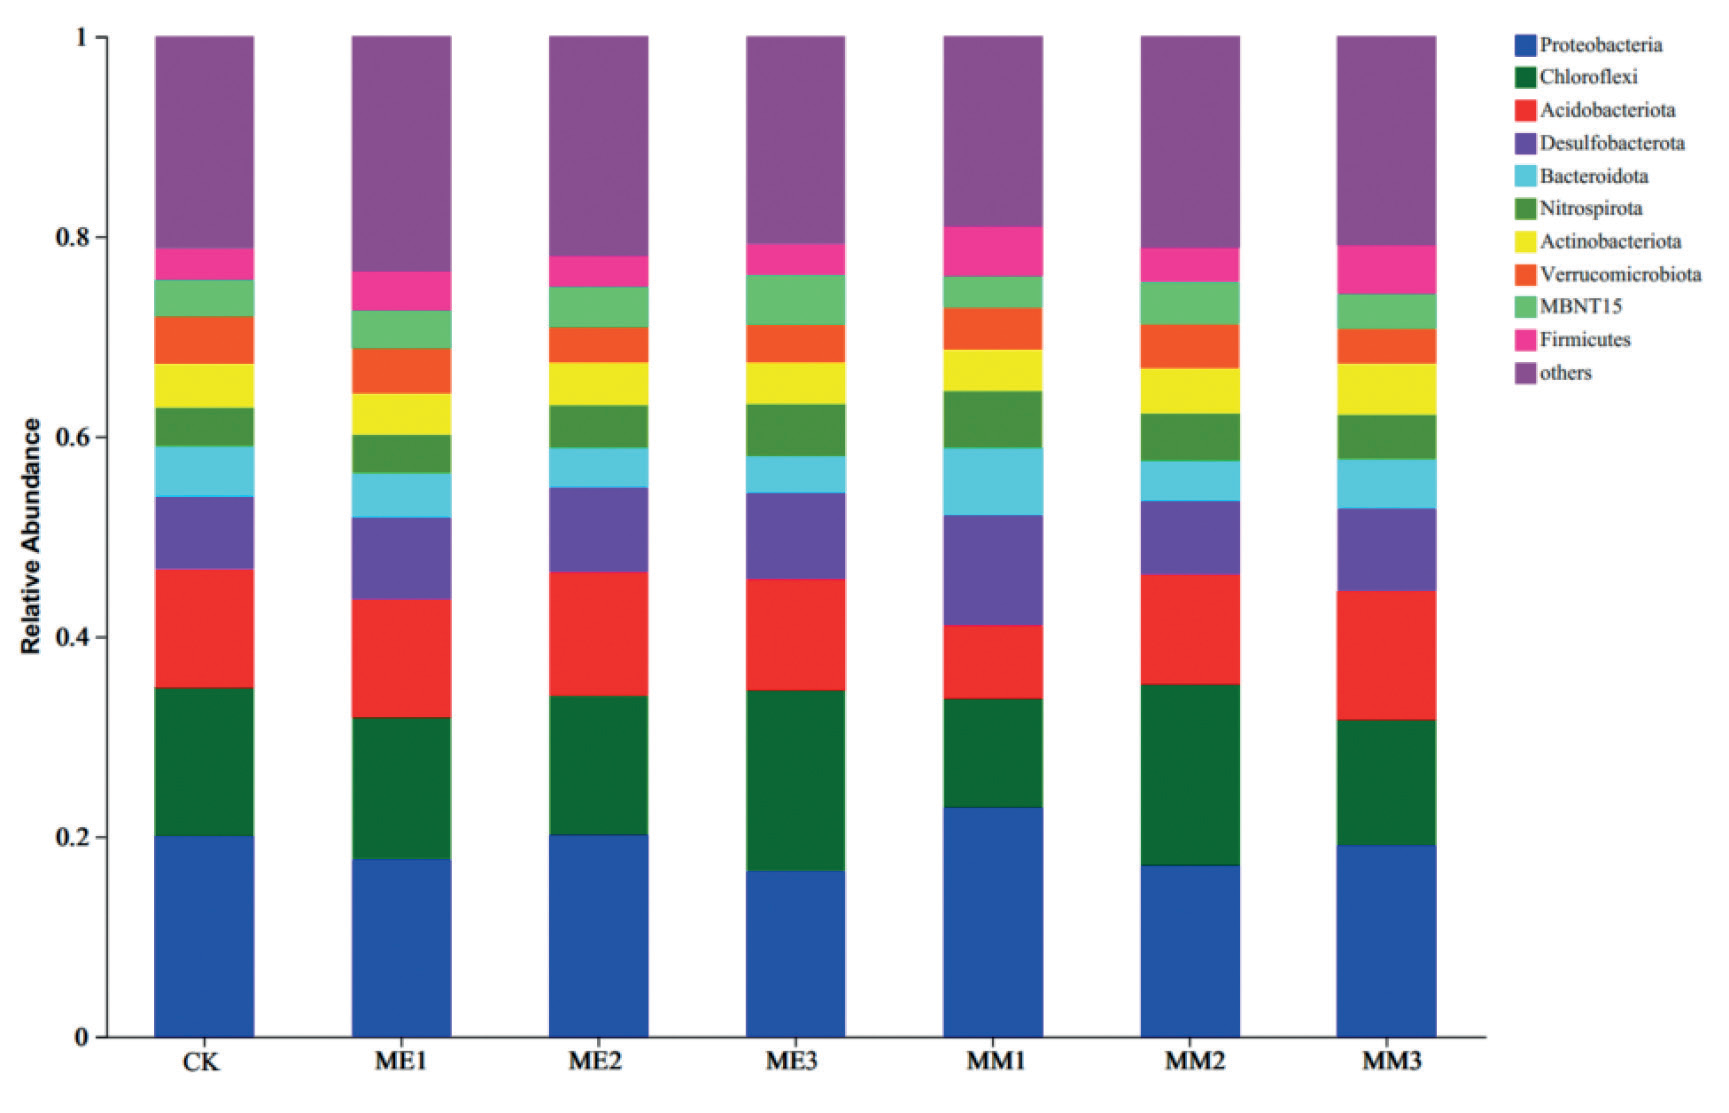
The dominant microbial species in each group were similar (Fig. 6). Among the observed phyla, Proteobacteria, Chloroflexi, Acidobacteriota, Desulfobacterota, and Bacteroidota were prevalent in all samples, constituting the top five bacterial groups, and accounting for >51% of the total abundance in order of occurrence. With substrate addition, the proportion and composition of dominant bacteria varied. Except for the ME2 and MM1 groups, the relative abundance of Proteobacteria was lower in the treatment groups than in the CK group (20.04%). Further, the relative abundance of Chloroflexi in the ME3 and MM2 groups exceeded that in the CK group, whereas the other treatment groups exhibited the opposite trend. Moreover, the relative abundances of Desulfobacterota and Nitrospirota communities in each treatment group exceeded those in the CK group.
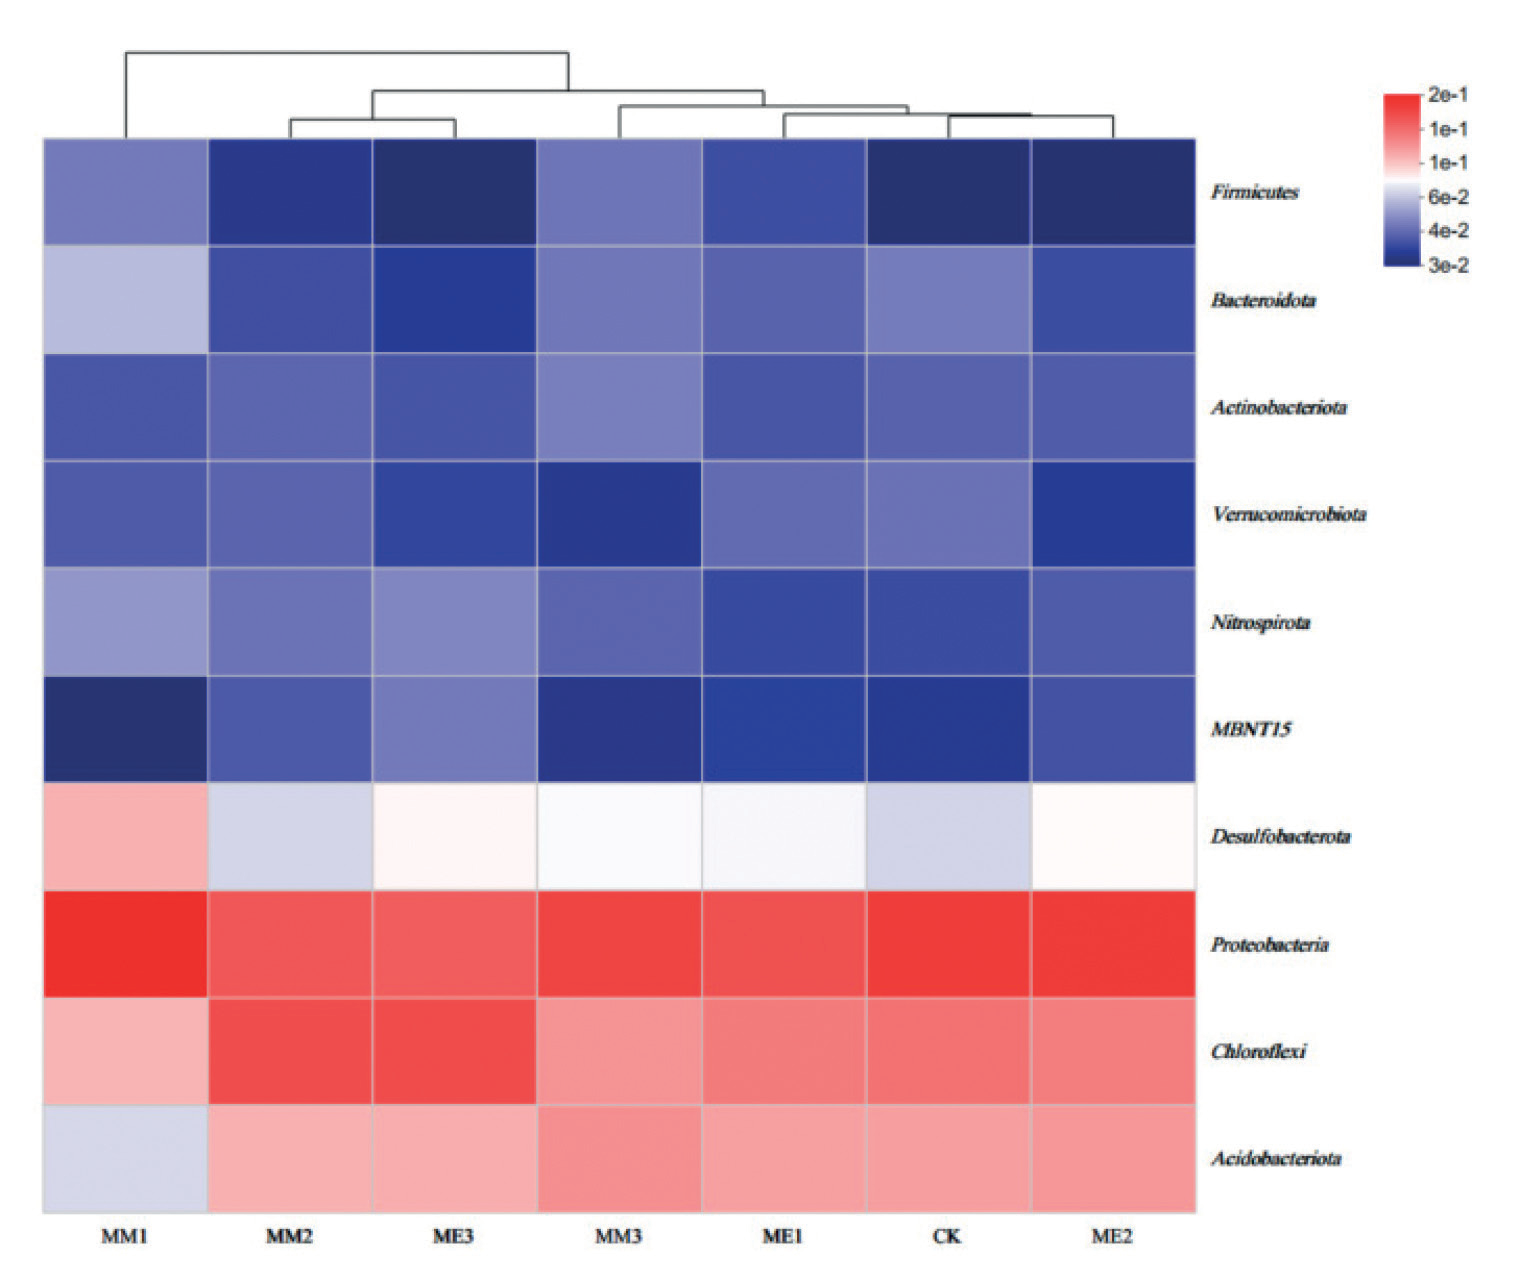
In Fig. 7, the heat map of the clustering tree illustrates the similar and different microbial composition in each sample under various treatments. Following cluster analysis, the microbial community was divided into three branches: MM3 and CK, ME1, and ME2 formed a branch; MM2 and ME3 formed a branch; and MM1 formed a separate branch. Additionally, MM1 formed a distinct branch, indicating a distinctly distant microbial evolution relationship between the MM1 group and other group samples.
Discussion
Previous studies have reported a correlation between substrate type and the growth of submerged macrophytes [21, 22]. For instance, the addition of maifanite to sediments significantly enhances the growth of Hydrilla verticillata [23], with the relative growth rate of V. natans increasing by up to 163.1% upon the addition of biochar [24]. In the present study, various treatments exerted significant positive effects on the growth of V. natans (Fig. 2). This can be attributed to the enhanced sediment porosity and permeability resulting from substrate addition, thus promoting growth [25]. Accordingly, the average biomass growth rate of V. natans in the treatment group exceeded that in the CK group at 120 days. In the later stages of cultivation (90–120 days), the number of leaves and root length significantly increased in the MM2 and MM3 groups compared with the unmodified maifanite groups. This may be attributed to the higher concentration and rate of Mg2+ released by the modified maifanite compared with the unmodified maifanite. These Mg2+ ions accelerate the transport of carbohydrates from source to sink within the plant [26], enabling the rapid absorption of nutrients and growth acceleration. Similar to these results, Koch et al. reported that Mg transport plays a crucial role in plant growth and that under Mg-deficient conditions, plants interrupt this transport process, significantly reducing the root and stem growth rate [27].
MDA is a byproduct of the oxidative degradation of membrane lipids and its accumulation reflects the degree of lipid peroxidation in plant cell membranes and their adaptability to environmental changes [28]. Higher MDA accumulation indicates greater damage to the plant cell membrane [29]. In our study, the MDA content in the CK group was higher than that in the treatment groups, indicating that the presence of substrate mitigated oxidative damage to submerged macrophyte leaves. Chen et al. [30] also observed that plant growth is heavily dependent on substrate, with the lack of substrate exerting a substantial stress on plant growth. Throughout the experimental period, the MDA content in the modified maifanite groups peaked earlier than that in the unmodified maifanite groups, suggesting that the addition of Mg2+ can accelerate the adaptability of V. natans to changes in the external environment.
Under stress, the dynamic equilibrium of reactive oxygen species within plant cells can be disrupted [31]. In such conditions, plant cells generate endogenous antioxidant enzymes, such as SOD and CAT, to eliminate the excess reactive oxygen species [32]. In the present study, following substrate addition, the SOD and CAT activities remained elevated in the early cultivation stage (30–60 days), peaking earlier than in the CK group. This suggests that after the transplantation of V. natans, numerous reactive oxygen species were produced in V. natans leaves, and substrate addition facilitated the rapid production of antioxidant enzymes to remove these oxygen radicals. Throughout the experimental period, the average CAT activity in the leaves tended to initially increase and then decrease with the increase in substrate. This observation is consistent with the findings of Liu et al. [22], who reported that excessive substrate addition could increase growth pressure at the base of the plant stem, thus inhibiting plant growth. Mg2+ is a key component of the enzymes involved in carbohydrate metabolism; it plays a crucial role in activating enzymes and can effectively promote enzymatic reactions closely related to cell material synthesis [33]. Therefore, at the same dosage, the average CAT activity in V. natans treated with modified maifanite was higher than that in V. natans treated with unmodified maifanite.
Fig. 6.
Effects of different treatments on the structure composition and relative abundance of dominant microbial phyla in the rhizosphere of V. natans.
The root vitality of plants directly influences their growth and development [34]. In the present study, root vitality was positively correlated with chlorophyll and plant growth indices, with the MM2 group exhibiting the maximum increase in root length at the end of the culture period. These findings indicate that Mg2+ could enhance the oxidation activity in roots, promote cell division, and elongate the root tip meristem, thereby protecting root ultrastructure and alleviating the impact of external stress on plant roots [35].
Our findings revealed that substrate addition did not alter the dominant microbial phyla in the rhizosphere but did affect the α-diversity and relative abundance of these microorganisms. Following substrate addition, the relative abundance of the Desulfobacterota and Nitrospirota phyla in the rhizosphere increased. These are crucial species involved in sulfur and nitrogen cycling in sediments [36, 37] and can directly engage in reactions such as electron transfer, oxidative stress response, and nitrogen fixation because of the gradual release of nutrients from the substrate [17]. This makes these microbial groups more competitive in adapting to the altered environment. Additionally, in our study, the microbial diversity in the modified maifanite group exceeded that of the other groups. This phenomenon may be attributed to Mg2+ which serves as a cofactor for various enzymes and can participate in multiple metabolic processes in microorganisms. This promotes the growth and activity of aquatic microorganisms while preserving the richness and diversity of microbial communities [38, 39].
Conclusions
In this study, we used different dosages of modified and unmodified maifanite and assessed the growth of V. natans and changes in rhizosphere microorganisms under these doses. Our results highlighted significant differences in the increase in height in each group throughout the cultivation period, with the MM2 group exhibiting the maximum increase of 50 cm. The root length of V. natans in the modified maifanite groups exceeded that in the CK group at each time point, whereas the MDA content in the leaves in the CK group was consistently higher than that in other groups, with significant differences. For the entire culture period, the mean CAT activity in leaves first increased and then decreased with substrate dosage. These findings indicate that substrate addition could enhance stress resistance in plants, with excessive addition affecting the transformation of related enzymes in V. natans. The diversity and abundance of rhizosphere microorganisms in modified maifanite groups exceeded those in other groups, with the MM2 group exhibiting the highest values. Overall, this study demonstrated that the addition of modified maifanite in sediments was more conducive to the growth of submerged macrophytes and the reproduction of rhizosphere microorganisms compared with unmodified maifanite, with the optimal dosage identified as 400 g m-2. These results provide a scientific basis for the screening of sediment substrate modifiers.

