

Introduction
Elevated soil acidity and alkalinity are stressful conditions for plants, which mainly affect their growth rate. Soil pH determination and the integral chemistry of plant nutrient colloidal solutions are regulated by H+ ion concentrations. PH-induced toxicity, nutrient imbalance, metal level enrichment, and deficiencies are multiple stresses that generally affect the soil, plant, and environmental continuum [1-3]. Natural weathering processes or sometimes man-made conditions (e.g., irrigation practices) also cause alkalinity stress. Sometimes the neutralization process occurs because of the high concentration of carbonates (CO32–) and bicarbonates (HCO3–) which can neutralize the soil acids. As a result, in most areas of the world, both soil alkalinity and salinity are associated with desertification [4, 5]. Global wheat production is intricately influenced by a complex interplay of biotic and abiotic factors, which collectively shape the yield, quality, and overall sustainability of this crucial staple crop. Biotic factors, encompassing pests, diseases, and pathogens, can lead to substantial yield losses [6]. Similarly, abiotic factors such as temperature extremes, drought, soil quality, and nutrient availability play a pivotal role. Additionally, water scarcity, soil degradation, soil salinity, or alkalinity can hinder wheat’s growth and nutrient uptake, limiting its potential yield [7]. Generally, increased salt concentrations inhibit germination, but alkaline stress has an even stronger effect on wheat crops. The effect on the roots was more significant in comparison to alkaline stress and saline stress [8, 9]. Alkaline stress has a pronounced effect on photosynthetic components and the chloroplast structure. [10]. Proline and glycine betaine are regarded as compatible solutes within the cytoplasm of cells. Sodium ion (Na+) deficiency in the mesophyll tissue of plant leaf cells caused by salinity promotes a net reduction in the photosynthesis of plants. The oxidative stress rate is also affected by salinity and alkalinity, which lead to the damage of cells, proteins, lipids, and nucleic acid [11].
Wheat is indeed the most important staple crop, with roughly 720 million tons produced worldwide. Wheat yields must be raised to fulfill the rising population’s food demands and long-term food security due to climate change. The development of alkaline-tolerant cereals (wheat and rice) genotypes with significant adaptive and agronomic features is critical for wheat growers. For enhanced adaptation to changing climatic circumstances, selection should normally target genotypes with relatively high yields under both stressed and optimal conditions. So, the exploration of morphophysiological, biochemical, and enzymatic antioxidants and ionic homeostasis under alkaline stress in diverse cultivars at the early seedling stage is necessary when breeding for alkalinity tolerance, as linked to yield and its component traits will be very beneficial. The selection of cultivars for stress, coupled with acceptable agronomic procedures, has been a suitable way to deal with abiotic stresses in agriculture [12]. Therefore, the objectives of this study were 1) to estimate the range of variability in the morphophysiological, biochemical, enzymatic antioxidants, and ionic homeostasis in the wheat cultivars under three contrasting alkalinity regimes, and 2) to identify wheat cultivars that are tolerant and resistant to alkalinity stress at early seedling growth.
Materials And Methods
Plant Materials
This research work was carried out at the environmental analytical laboratory, Department of Environmental Sciences, University of Lahore, Pakistan. The healthy seeds of five wheat cultivars (Akbar 2019, Anaj 2017, Zincol 2016, Punjab 2011, and FSD 2008) were obtained from the Ayyub Agriculture Research Institute (AARI) in Faisalabad, Pakistan, and stored in paper bags at room temperature (20±2ºC).
Experimental Setup and Maintenance
The experiment was conducted in a completely randomized design (CRD) with five replications under the factorial arrangement where the treatments were assigned completely at random and comprised of two factors of alkalinity stress (0mM, 40 mM (NaHCO3 and Na2CO3 in a 9:1 molar), and 80 mM (NaHCO3 and Na2CO3 in a 9:1 molar). The seeds were surface sterilized in 0.1% HgCl2 for two min, and 10 seeds were sown in each petri plate between two layers of moist filter paper. Samples were placed in growth chambers (HPG-400, Harbin, China) with a 16-h photoperiod. The temperature was 25±2ºC during the day and 21±1.5ºC during the night. The seedlings were treated using Hoagland’s solution containing polythene sheets, which were also lined during two leaf stages [13]. A supply of bubbling air through the nutrient solution for 8 h daily was carried out as part of aeration for sample preparation. After one week of transplanting, alkalinity between 40 and 80 mM was developed stepwise, whereas in the control condition, alkalinity was not developed. The EC (1.53, 4.25, and 8.25 dS m-1) and pH (6.92, 8.75, and 9.50) of the stress treatment solution for control were 40 mM and 80 mM, respectively. After 45 days of the imposition of alkalinity stress, plants were harvested at their maturity level.
Data Collection
After the plants were harvested, they were washed, and the lengths of roots and shoots were measured. The fresh seedling biomass was also measured. Seedlings were desiccated in an oven at 65ºC until their weight was constant, and their dry weight was determined.
Non-Enzymatic and Physio Biochemical Attributes
The SPAD chlorophyll values were determined using the SPAD 502 Plus Chlorophyll Meter (Minolta, Ramsey, NJ). Subsequently, photosynthesis related measurements were conducted between 9:00 a.m. and 11:00 a.m., ten days following the imposition of alkalinity stress. These calculations were taken using an IRGA (Analytical Development Company, Hoddesdon, England). To determine the relative water contents (RWC), the fresh and healthy leaves of wheat cultivars were placed in a plastic bag in order to reduce any potential water loss. The fresh weight of leaves from each treatment was determined using a weighing balance. To obtain the turgid weight leaves from each treatment were soaked for approximately 4-6 hours. After recording turgid weight, place the leaves from each treatment of the wheat cultivars into an oven at 60-70ºC until complete dryness. This drying process is necessary for estimating the dry weight of the leaves.
RWC measurements were done by following the method of Turner and Kramer [14], as mentioned in Equation (1):
Where FW, TW, and DW stand for fresh weight, turgid weight, and dry weight.
Electrolyte leakage (EL) was computed using a formula developed by Lutts and Guerrier [15], as described in Equation (2).
The proline contents were estimated by following the protocol of Bates et al. [16] using the acid-ninhydrin method. By using the standard linear curve (y = mx + b), the unknown value of proline content was determined. The total amount of proline content (PC) in a given sample is expressed on a fresh weight (FW) basis using the following formula [17], as mentioned in Equatio n (3).
where y = absorption at 520 nm; X = unknown concentration determined from the standard curve; m = slope; and b = y intercept. For the quantification of MDA (Malondialdehyde) contents, a fresh leaf sample (~0.5 g) of the plant was used in the thiobarbituric acid (C4H4N2O2S) reaction method [18]. The ascorbic acid determination protocols of Mukherjee and Choudhuri [19] were followed. For the estimation of total soluble sugars (SS), the anthrone reagent method was used at 70ºC in 70% alcohol for 30 min.
Enzymatic Antioxidants Attributes
The fresh leaf sample (0.25 g) was blended with 5 mL of potassium phosphate buffer (pH~7.8) and uniformly mixed after 15 min of centrifugation at 12,000 rpm and 4ºC. The extracted material was frozen at -20ºC for further analysis. Superoxide dismutase (SOD) activity was determined by calculating the inhibition of nitroblue tetrazolium (NBT) photoreduction using a spectrophotometer.
In a similar pattern, catalase activity was determined by following the method reported by Maehlys and Chance [20]. To determine peroxidase activity, sample extract (0.05 mL), H2O2 (0.1 mL), 1 mL reaction mixture, phosphate buffer (0.75 mL), and guaiacol (0.1 mL) were combined to prepare the mixture. After that, spectrophotometer readings were taken at 470 nm as the final value for the POD activity. The cations (Ca2+, Na+, and K+) concentration in roots and shoots was determined by following the method of Gorham et al. [21].
Criteria for the Classification of Wheat Genotypes for Alkaline Tolerance
Based upon the growth, biomass (fresh and dry), and ionic accumulation (leaf Na+, K+, and Cl- of leaf sap) attributes, all the genotypes were divided into the sensitive, moderately tolerant, and tolerant categories [21]. The values at two alkalinity levels (40 mM and 80 mM) were averaged.
It will be counted as the tolerant group if the average percent of control conditions at two alkalinity levels is ≥50% of the shoot fresh weight genotype. Those having values of 40-49.9% and <40% average of control condition percent at two alkalinity levels were considered moderately tolerant and sensitive, respectively. Similarly, both shoot dry weight and root fresh weight genotypes are categorized into the sensitive group, a moderately tolerant group, and a tolerant group, which has an average percent of control at two alkalinity levels of <55%, 55-69.9%, and ≥70%, respectively.
Results and Discussion
Alkalinity treatments significantly reduced the seedling growth and biomass attributes of wheat cultivars. For all the measured growth and biomass parameters of wheat plants, the negative effects of alkalinity stress at both levels in comparison with control were more severe in the FSD-2008 variety than the rest of the cultivars. Alkalinity stress at 40 mM and 80 mM reduced the root length of wheat plants by 20.05% and 46.07%, shoot length by 25.91% and 50.16%, root fresh weight by 30.84% and 41.79%, shoot fresh weight by 18.91% and 41.80%, root dry weight by 43.63% and 60.00%, and shoot dry weight by 20.28% and 46.95%, respectively, in comparison with the control. Under stress conditions, Akbar-2019 performed better than the rest of the cultivars and registered a lower reduction, followed by Anaj-2019 in seedling development and biomass attributes (Table 1). Cultivars were classified in alkaline tolerance criteria according to selection criteria based on shoot and root fresh weight and shoot dry weight, as given in Table 2. According to root fresh weight criteria, all the wheat cultivars were grouped under the moderately tolerant group, while for shoot fresh weight and shoot dry weight, all the cultivars fell under the tolerant group. But overall, Akbar 2019 showed more tolerance for alkalinity stress as compared to the rest of the cultivars.
Alkalization and wheat cultivars recorded significant differences in physio-biochemical and non-enzymatic attributes of wheat leaves (Table 1; Fig. 1). Under alkaline stress, all the physio-biochemical and non-enzymatic attributes in wheat cultivars were reduced compared to the control. Exposure to alkalinity stress at 40 mM and 80 mM reduced the chlorophyll content by 30.99% and 48.79%, the photosynthetic rate by 30.12% and 55.71%, the transpiration rate by 19.74% and 51.84%, the stomatal conductance by 44.89% and 81.63%, the relative water contents by 12.01% and 21.27%, and the total soluble sugars by 17.59% and 19.51%, respectively, as compared with control treatments. Compared with the control, alkaline stress at 40 mM and 80 mM increased the AsA contents by 23.22% and 32.25%, electrolyte leakage by 82.26% and 161.14%, free proline contents by 27.98% and 43.01%, and MDA contents by 16.42% and 30.52%, respectively. The wheat cultivar Akbar-2019, followed by Anaj-2017, recorded less reduction due to statistically being on par in chlorophyll content, photosynthetic rate, transpiration rate, stomatal conductance, electrolyte leakage, relative water contents, and total soluble sugars, as well as an improvement in AsA contents, free proline, and MDA contents under stress conditions.
The activities of antioxidant enzymes were significantly affected by alkaline stress treatments and wheat cultivars (Fig. 1). Alkaline stress enhanced CAT activity by 23.07% and 66.67%, SOD activity by 13.79% and 29.31%, and POD activity by 15.87% and 36.98% in 40 mM and 80 mM alkaline stress, respectively, compared with the control. The decreasing pattern in terms of enzymatic antioxidants for wheat cultivars was Akbar 2019>Anaj 2017>Zincol 2016>Punjab 2011>FSD 2008, and for alkalinity treatments, 80 mM>40 mM >control. Under alkaline stress conditions, the wheat cultivars Akbar-2019 and Anaj-2017 show increased activity of antioxidant enzymes due to statistically similar results in comparison to the rest of the cultivars.
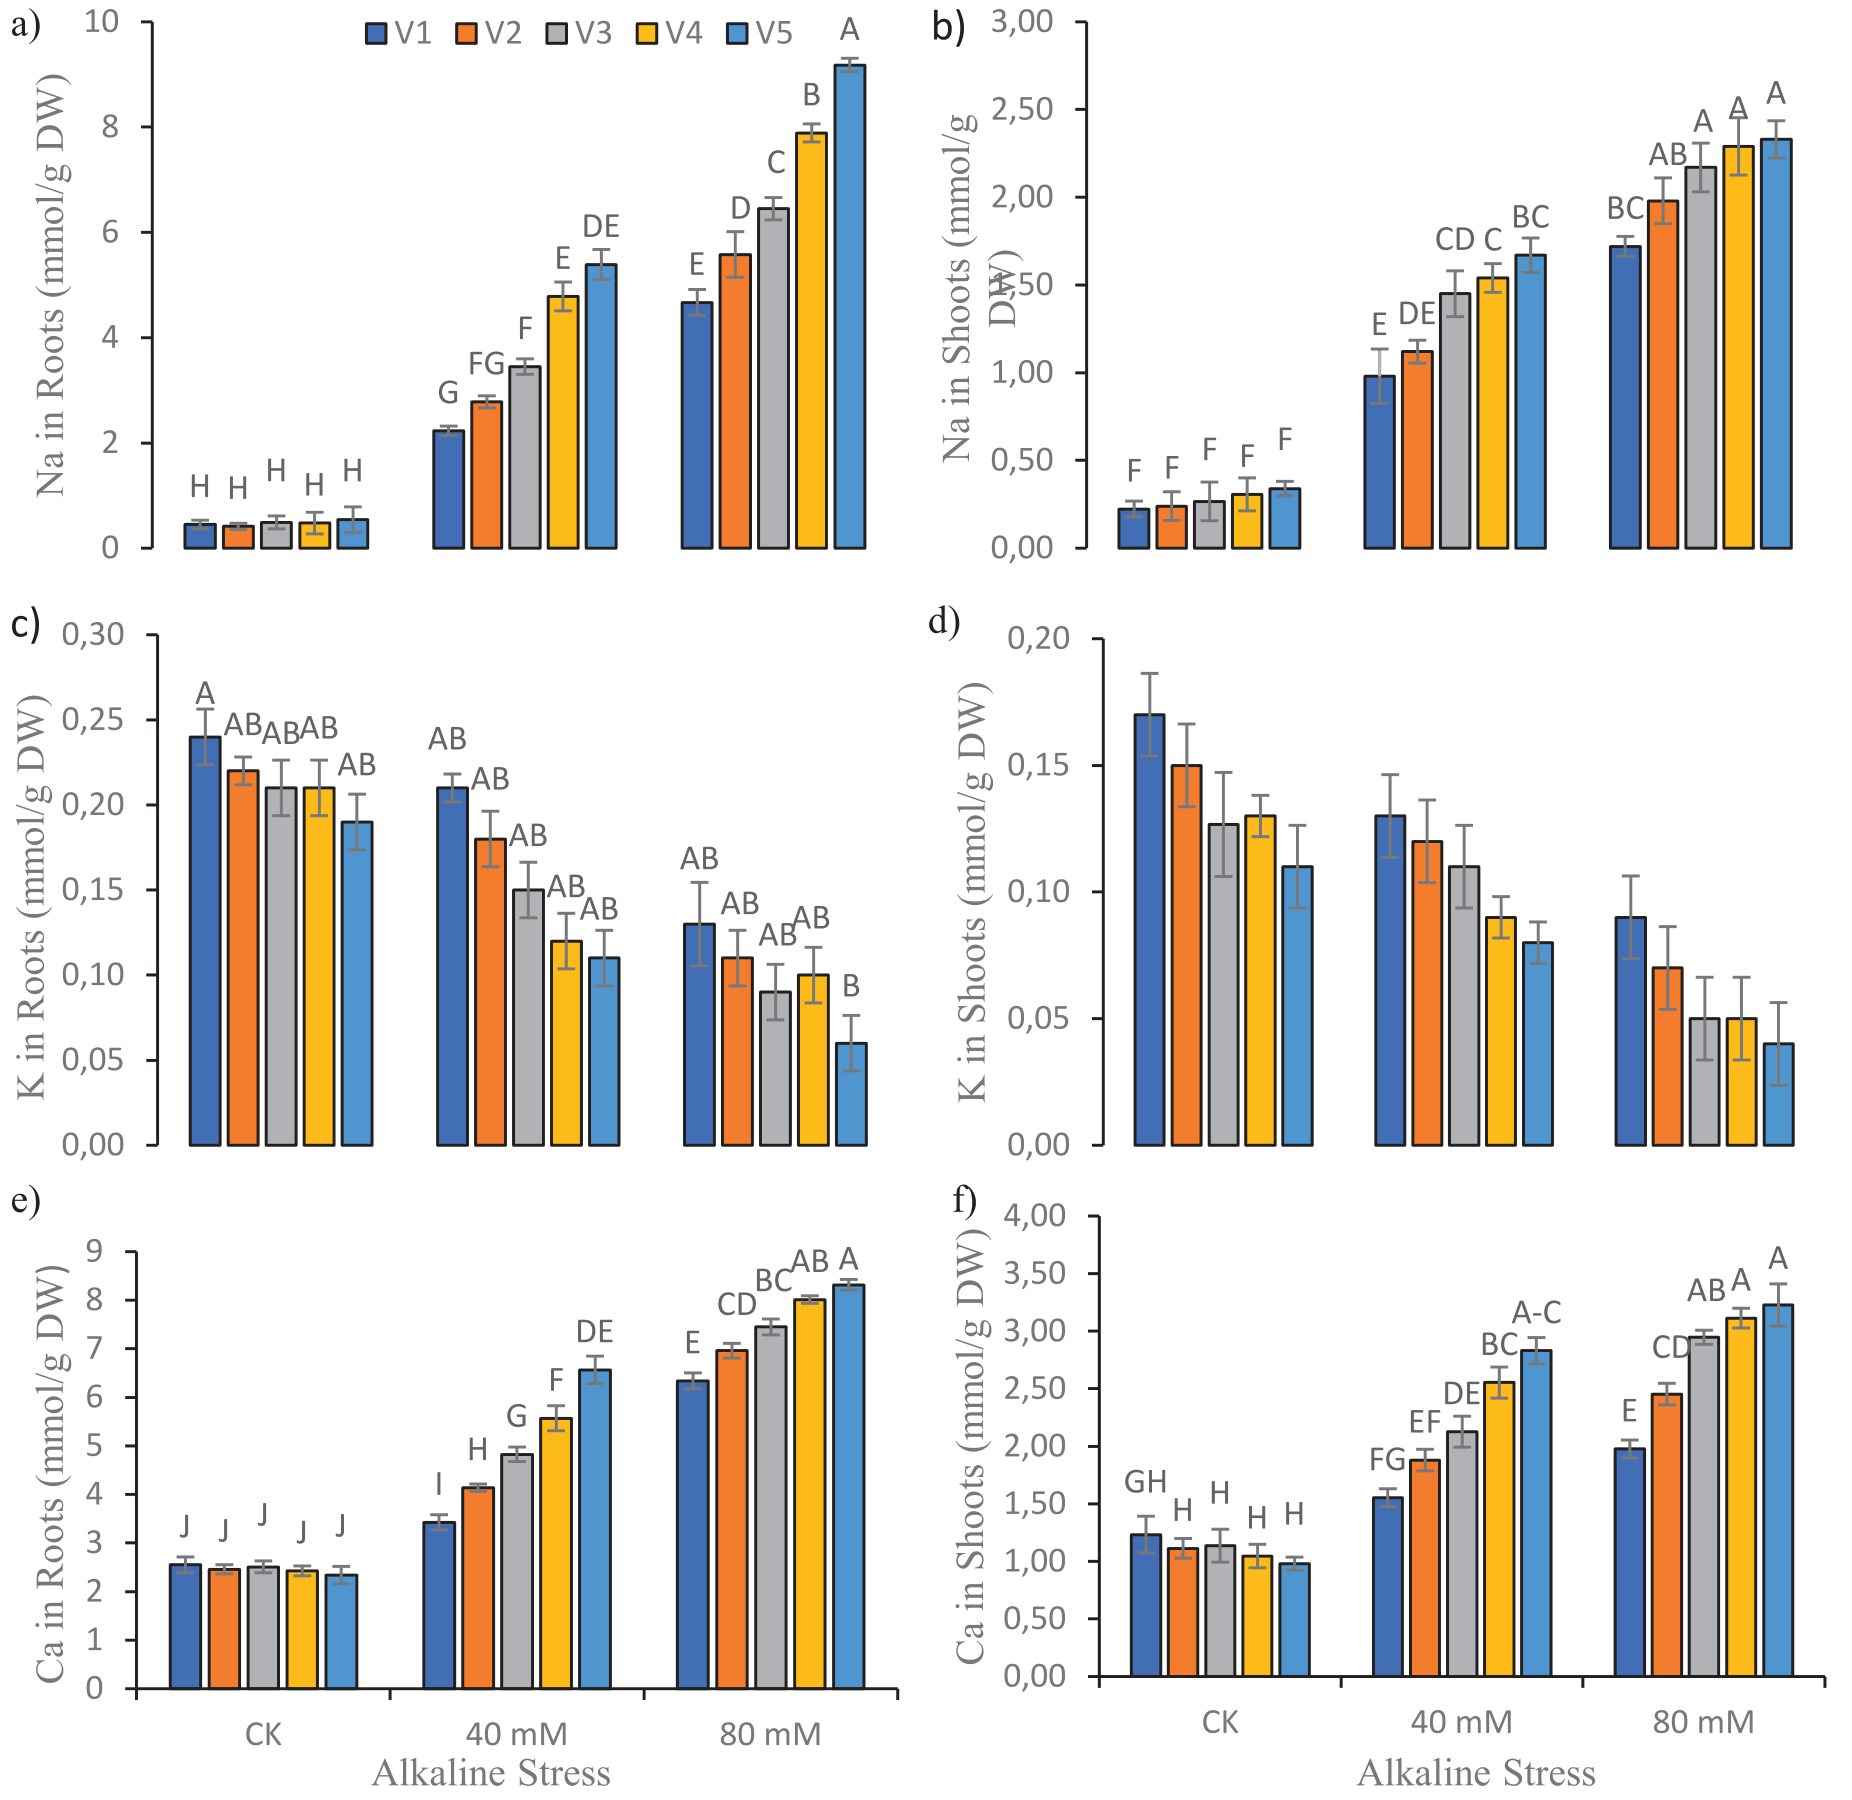
Alkaline stress treatments and wheat cultivars significantly affected cation accumulation in various plant parts except for the potassium contents in shoots (Fig. 2). Under alkalinity stress, the accumulation of K+ ions in all wheat cultivars was significantly higher than in the control. However, alkalinity-induced stress increased Na+ and Ca+2 ion levels in various plant parts of all wheat cultivars as compared to the control. Exposure to alkalinity stress at 40 mM and 80 mM increased the sodium and calcium contents in roots and shoots in comparison with the control. The wheat cultivars Akbar-2019 and Anaj-2017 were comparatively better than the rest of the cultivars and also in a stress condition due to better ionic balance maintenance.
Principal Component Analysis
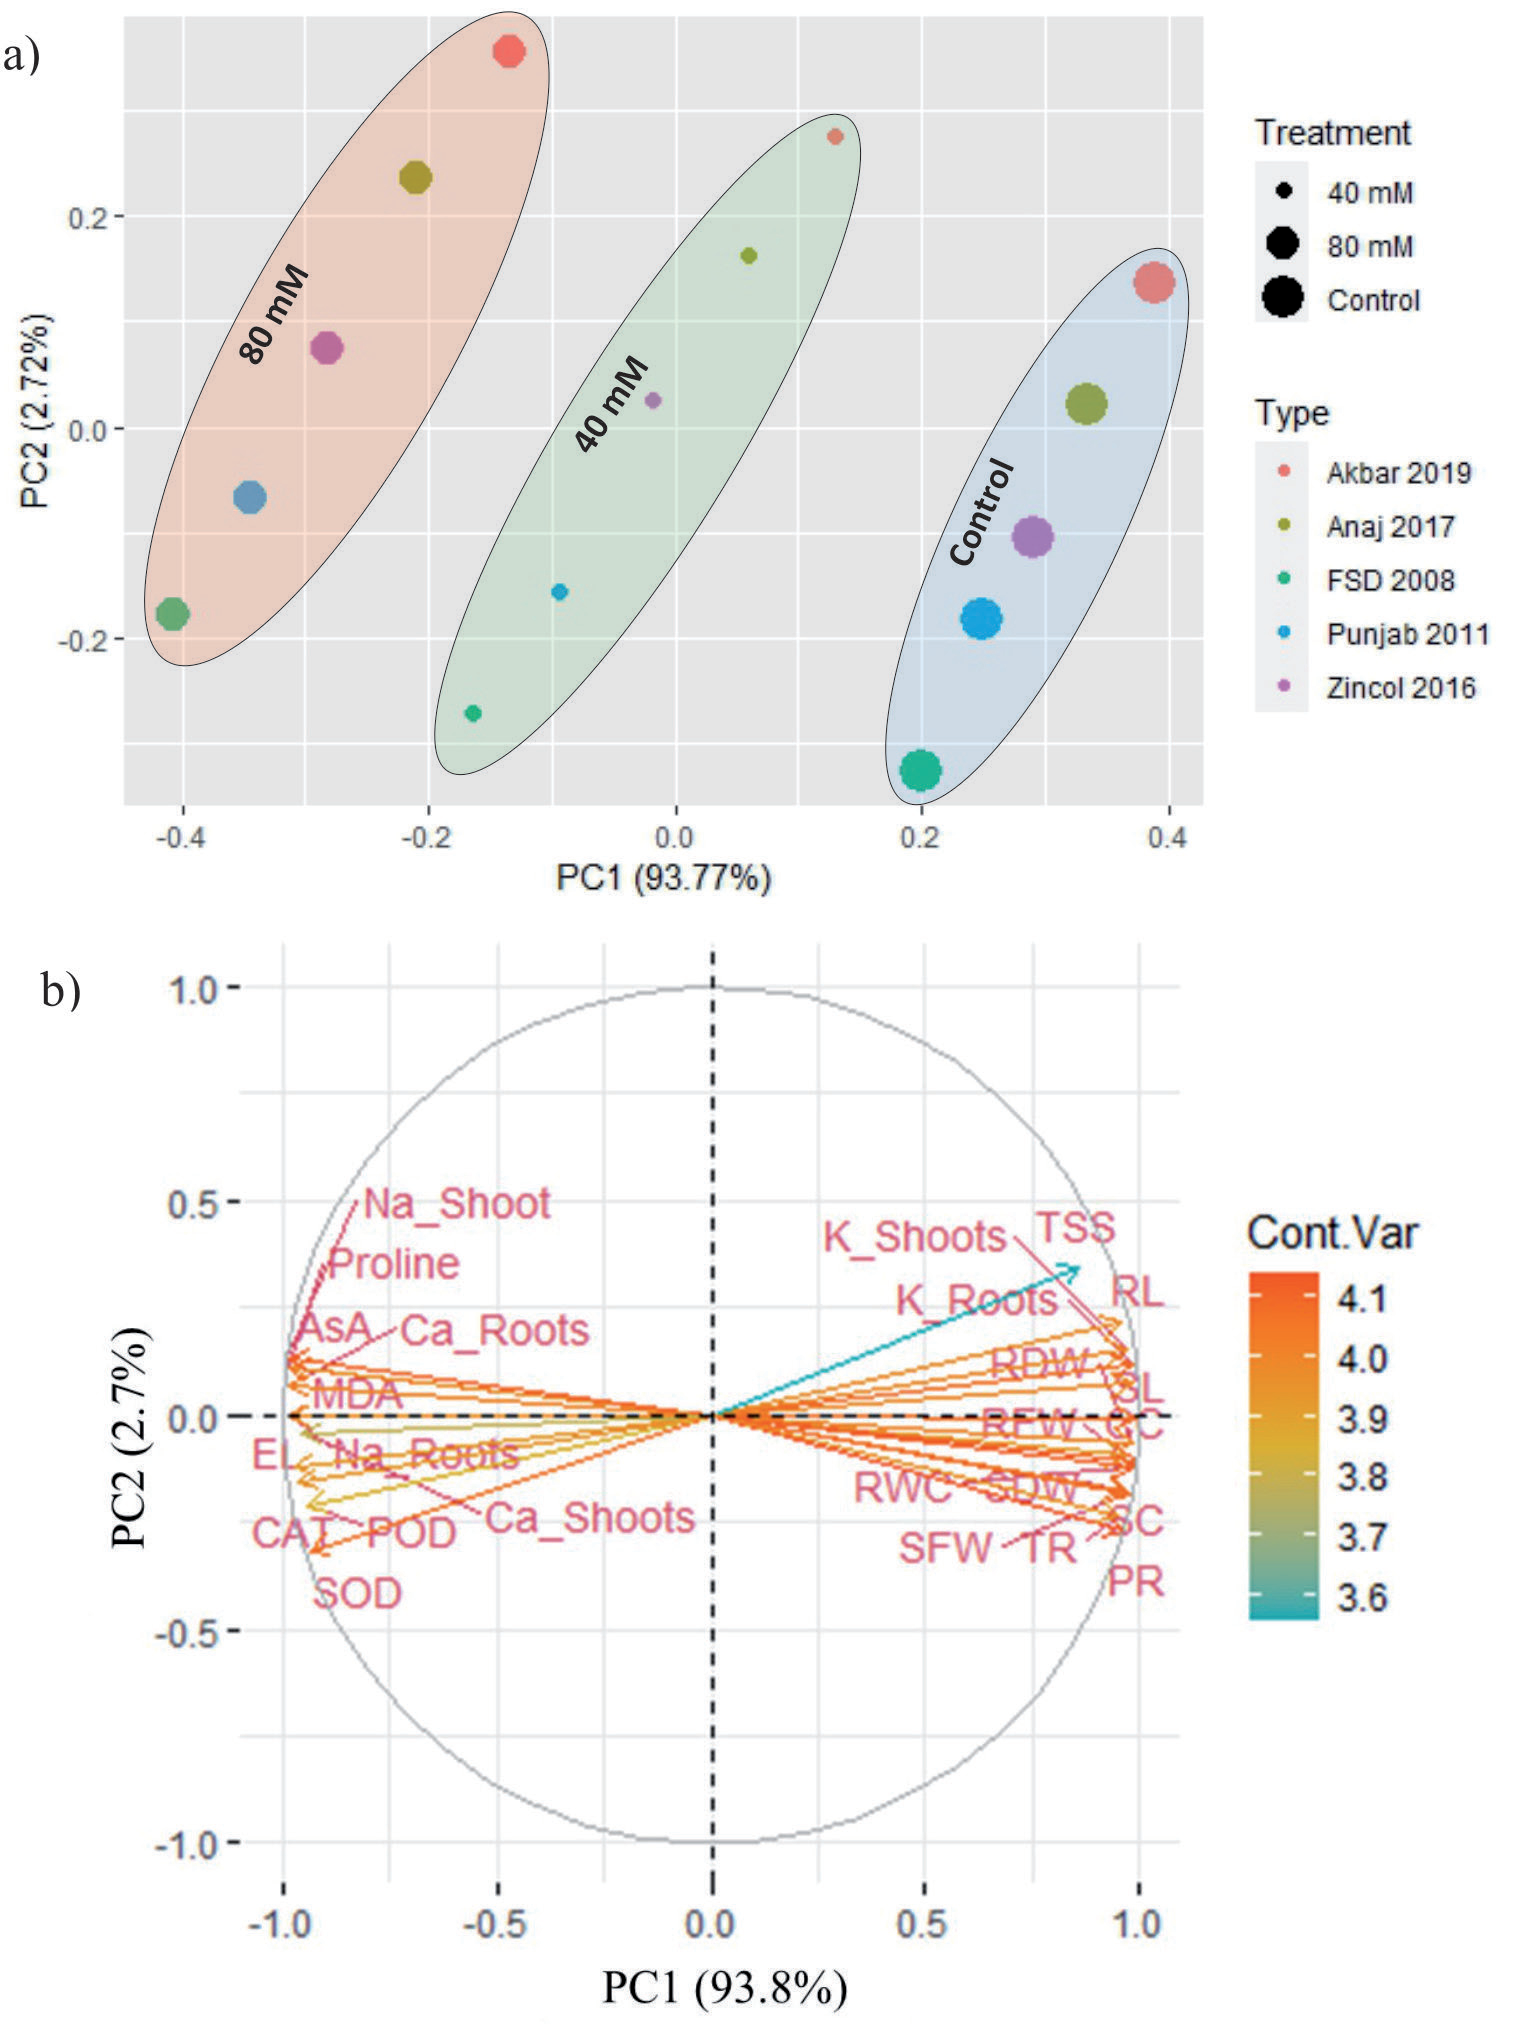
The Principal Component Analysis (PCA) is a multi-variate statistical technique that helps identify clusters of variables based on associations in all data sets [22]. The biplot and PCA analysis showed that the most distinguishing parameters, with positive vector loading in PC I, were total soluble sugars, root length, K in shoots, K in roots, shoot length, chlorophyll contents, root dry weight, root fresh weight, stomatal conductance, relative water contents, shoot fresh weight, shoot dry weight, transpiration rate, and photosynthetic rate. The genotypic variations with the treatment means can be determined by measuring the distance between the biplot origin and genotype (Fig. 3a and 3b). Thus, superior and inferior performers are the genotypes with maximum and minimum distances from the origin, respectively [23]. The two major clusters are on nearly opposite sides of the PC1 axis, depicting an inverse correlation among measured parameters. The two principal components (PC1 and PC2) are selected as the contributors to most of the variability (~96.5%) of the data. The RWC, SDW, and SFW, among others, indicated a stronger correlation among each other and an inverse correlation with MDA, proline, and Na in shoots, and others as shown in Fig. 3b). Proline contents serve several physiological functions in plants and are synthesized in response to these functions under stress-induced conditions. While the SFW and RWC contents are reduced when proline content is higher as part of and inbuilt defense mechanisms in plants.
High concentrations of alkaline salts or neutral salts affect wheat crop productivity [24]. This work examined the morphological, biochemical, physiological, and cationic status of the five wheat cultivars under alkalinity stress and clearly showed the effects of alkaline stress on the wheat cultivars’ oxidative metabolism and morphological processes.
Table 1.
Effect of various levels of alkaline stress (0 mM, 40 mM, and 80 mM) on the growth attributes, biomass, physio-biochemical and water-related of wheat cultivars.
[i] V1 = Akbar-2019; V2 = Anaj-2017; V3 = Zincol 2016; V4 = Punjab 2011; V5 = FSD 2008; RL = root length (cm); SL = shoot length (cm); RFW = root fresh weight (g); SFW = shoot fresh weight (g); RDW = root dry weight (g); SDW = shoot dry weight (g); CC = chlorophyll contents (mg L-1 FW); RWC = relative water contents (%); EL = electrolyte leakage (%); TR = transpiration rate (mmol H2O m-2 s-1); PR = photosynthetic rate (μmol CO2 m-2 s-1); SC = stomatal conductance (mmol H2O m-2 s-1); The different uppercase letters in column showed the significant variations across treatments means, while values sharing same letters are not statistically significant at p<0.05, values denote the means.
Table 2.
Root fresh weight response, shoot fresh weight response, and shoot dry weight response of different wheat genotypes at different alkalinity stress.
This study also shows alkalinity stress caused a significant reduction in the growth and fresh and dry biomass of root and shoot in wheat cultivars. At higher levels of alkaline conditions, the reduction in plant growth and biomass was significant as compared to the non-stressed control. Higher pH rates under alkaline stress might cause a significant reduction in biomass and growth. Plant growth is also affected by the ionic imbalance and toxicity of specific ions. For instance, rice’s root cell damage, and seedling development inhibition occur, which mostly lead to plant wilting, and in the end, death, which is most probably caused by the higher pH conditions [25]. The high accumulation of Na+ ions and low K+ ions in cells inhibits the growth process of the cells. Cell osmotic pressure is regulated by potassium ions, and cells cannot reach their maximum size due to their hard structure and lose their expansion pressure. It was observed that the application of salts enhanced the concentration of Na+ ions in maize roots and also showed a greater reduction in the biomass of maize plants. Shoot elongation is dependent more on plant genetic makeup and is not a promising parameter for measuring salt tolerance [26]. So, we emphasized shoot/root fresh and dry weights as well as chemical parameters for more effective screening.
Alkalinity stress enhances the chlorophyll-degrading enzyme activity and also reduces the total chlorophyll contents and physiological attributes [27]. The reduction in chlorophyll contents might be due to a reduction in the uptake and movement of Mg2+ concentration, which is the structural block of the central atom of the chlorophyll molecule. The degradation of green pigments is also due to the low Mg2+ concentrations. Hence, alkalinity decreases physiological attributes due to the high enzyme activity of chlorophyllase. In wheat, though the application of alkaline stress improved stomatal conductance by diminishing water uptake [28].
The optimal level of RWC in cells and tissues is associated with increased metabolic activity. Alkaline stress substantially suppressed the RWC of wheat plants in this study. Under alkaline stress, wheat plant tissues exhibited elevated levels of EL. These results demonstrated that under high alkaline conditions, membrane stability is reduced in comparison with the control under non-stressed conditions. Under alkaline stress, osmoprotectants such as proline and sugar accumulation protect plant cells by adjusting vacuoles and harmonizing the cytosol. The overproduction of ROS is another substantial process caused by abiotic stress in higher plants, as evidenced by the increased lipid peroxidation contents. These findings are consistent with other studies, such as those involving grapevine rootstocks [29] and maize plants [30]. The alkaline stress increases the malondialdehyde (MDA) and free proline contents.
Fig. 1.
Effect of various levels of alkaline stress on the enzymatic attributes a) malondialdehyde contents, b) free proline contents, c) superoxide dismutase, d) peroxidase activity, e) catalase activity, f) ascorbic acid contents, g) total soluble sugars of wheat cultivars. The uppercase letters in graphs showed significant variations across treatment means at p<0.05, values denote the means.
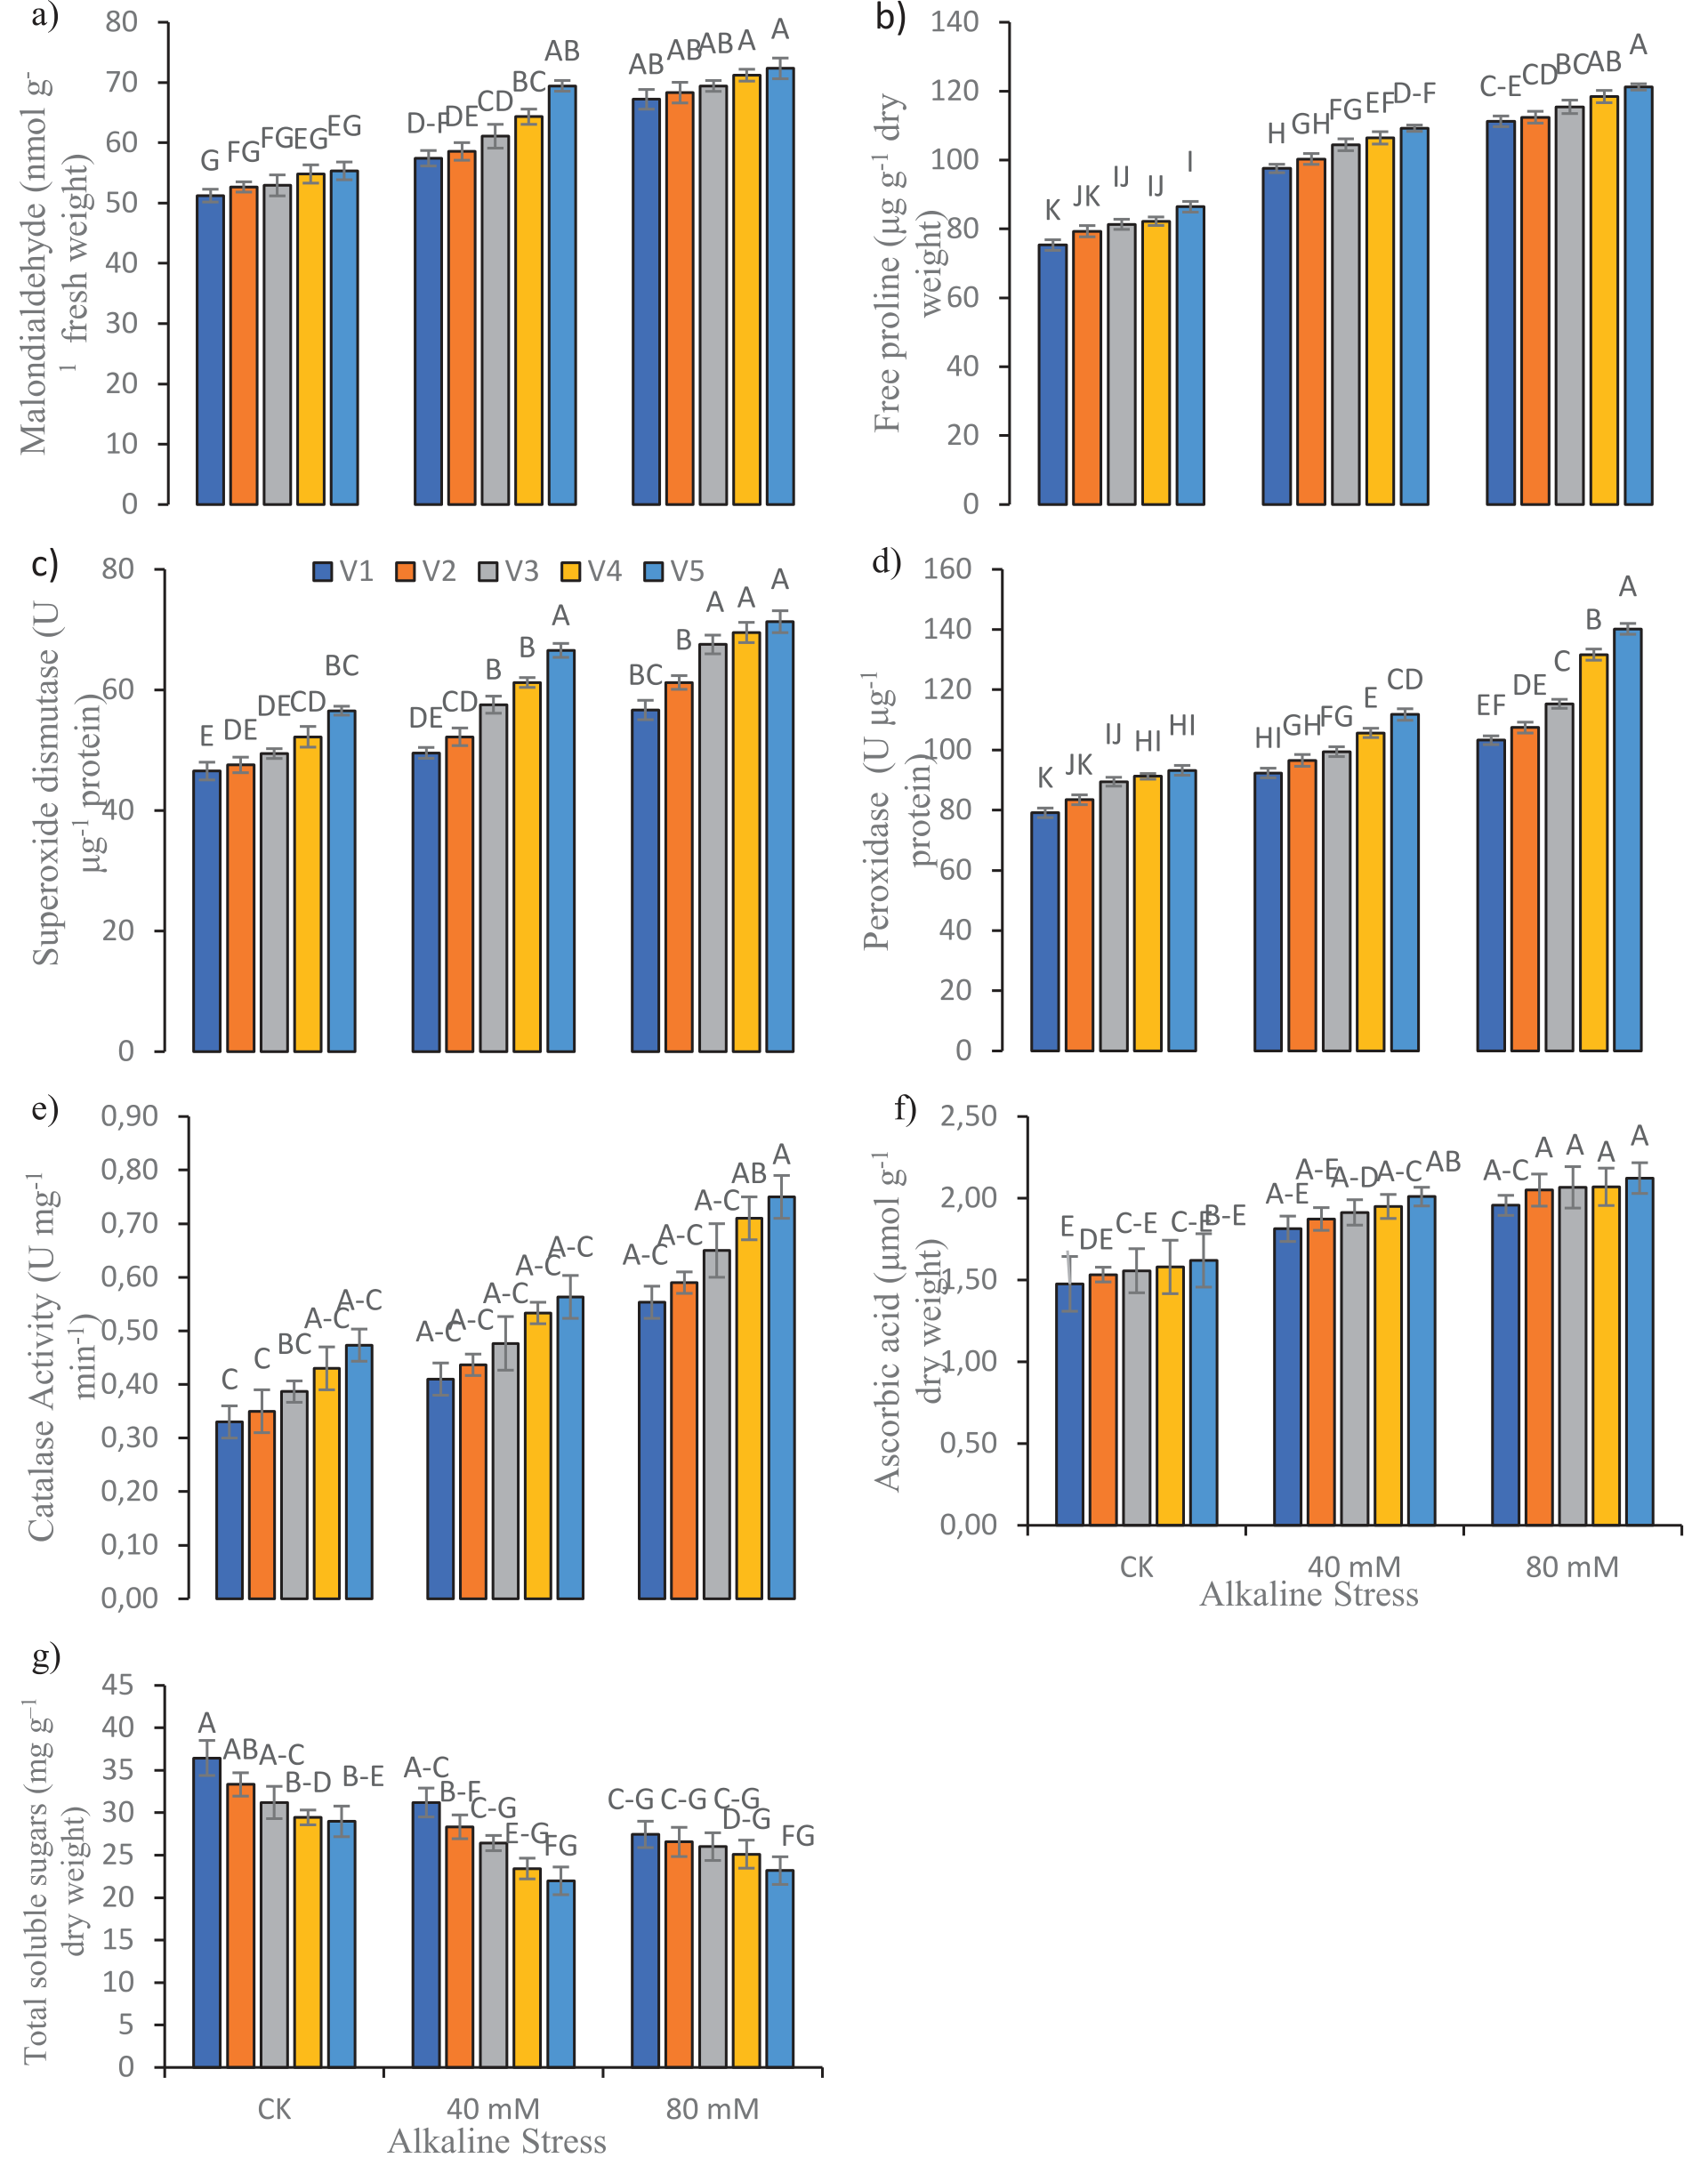
Fig. 2.
Effect of various levels of alkaline stress on the cations contents in various plant parts a) sodium contents in roots, B) sodium contents in shoots, c) potassium contents in roots, d) potassium contents in shoots, e) calcium contents in roots and f) calcium contents in shoots of wheat cultivars. The uppercase letters in graphs showed significant variations across treatment means at p<0.05, values denote the means. Figures without uppercase letters showed non-significant variation.
This study shows that at higher alkaline stress, some cultivars show positive responses for enzymatic antioxidants. Antioxidant enzymes deal with oxidative stress, which is produced in large quantities by wheat-tolerant varieties. The activities of SOD, CAT, and POD are significantly regulated under alkalinity conditions, as indicated by the data collected in this study. The regulation of SOD in plant development depends on environmental and tissue-specific signals. After SOD dismutation of O2− to H2O2, further dismutation of H2O2 takes place in the peroxisomes by CAT. At the reproductive and vegetative stages, the concentration of CAT increased in pearl millet plants due to salt stress [31]. SOD dismutation of O2− in chloroplasts produced the POD decomposition of H2O2.
In the present study, alkalinity-induced stress increased Na+ and Ca+2 ions while decreasing the K+ ion concentrations in the various parts of wheat cultivars (Fig. 2). Sodium is the main toxic and inorganic ion in alkaline conditions, so an ionic imbalance in cells is largely due to the accumulation of sodium. The increase in alkaline toxicity inhibits the absorption of potassium ions and the accumulation of Na+ ions in plants. The exchange capacity of the Na+/K+ ions is reduced due to salinity and alkalinity stress and also due to a low amount of sodium exclusion on the external side of the cell, resulting in higher cation accumulation [32]. Therefore, sodium ion levels in the roots and shoots are high in all wheat cultivars due to the low concentrations of sodium outside the cell. Osmotic stress is not only the reason for the high concentration of Na+ in the cells, but high pH also causes specific ion toxicity. The imbalance of sodium and potassium ion concentrations due to high pH, reduces the capacity of roots to absorb cations in alkaline settings. The ionic imbalance is caused by the sharp reduction of K+ ions in plant shoots under alkalinity stress.
Fig. 3.
Biplot (Principal component analysis) for all attributes measured in wheat cultivars under alkaline stress (40 mM and 80 mM) and control conditions.) Scatter plot, ) loading plot showed the distribution of five wheat cultivars for growth, physio-biochemical, non-enzymatic, and enzymatic antioxidants. Three distinct groups based on the levels of applied treatment and the control. The 40 mM level group plots in the middle of the 80 mM and the control group. The first two primary components, PC1 and PC2, make up the largest percentage of all components and account for more than 96% of the entire database. PC1 makes up 93.2% of this dataset, whereas PC2 makes up 2.7% of it. The figure represents the variation of genotypes with respect to the correlation. More the deviation from the center more will be the tolerance ability of the genotype. Akbar-2019 showed a positive response (alkalinity tolerant) in terms of alkaline stress and showed little variation as compared to FSD-2008 (alkalinity sensitive) which showed that the alkalinity stress significantly affected it as compared to control. All the growth, biomass, and physiological attributes are positively correlated with each other, while the antioxidants and ionic status of all the genotypes were negatively correlated with each other. RL = Root length; SL = Shoot length; RFW = Root fresh weight; RDW = Root dry weight; SFW = Shoot fresh weight; SDW = Shoot dry weight; CC = Chlorophyll contents; TR = Transpiration rate; SC = Stomatal conductance; PR = Photosynthetic rate; RWC = Relative water contents; SOD = Superoxide dismutase activity; POD = Peroxidase activity; CAT = Catalase activity; EL = Electrolyte leakage; MDA = Malonaldehyde contents; TSS = Total soluble sugars; AsA = Ascorbic acid; Na-Roots = Sodium contents in roots; Na-Shoots = Sodium contents in shoots; K-Roots = Potassium contents in roots; K-Shoots = Potassium contents in shoots; Ca-Roots = Calcium contents in roots; Ca-Shoots = Calcium contents in shoots;
Conclusions
Growth parameters like fresh and dry biomass and roots were found to be more important for screening germplasm against alkalinity at early growth stages and shoot developments. Alkalinity stress reduced the growth rate and biomass of all the wheat cultivars, disrupted the balance of ions, enhanced the rate of lipid peroxidation, and regulated the antioxidant enzyme activities. Alkalinity stress of all traits showed a negative effect far more severe in the FSD-2008 wheat variety. Under alkaline stress conditions, Akbar-2019 proved to be a better survival variety than the rest of the cultivars by showing less reduction in biomass and growth. The Akbar-2019 performance is most likely associated with higher antioxidant enzyme activity, photosynthetic pigment maintenance, and ionic balance under alkalinity stress and, hence, should be preferred over other varieties in alkalinity-induced stress soil environments.

