

Introduction
Camelina sative is called false flax, which is a low-input crop currently researched as an alternate oilseed crop [1]. This species is grown in a waste area of the world as it has high productivity, needs low input, is tolerant to cold weather and a short growing season, and is well grown under semi-arid conditions [2]. It is used in the production of biofuel, biopolymers, and cosmetics [3]. It also has the potential for edible oil due to its unique fatty acids [4]. Having several agronomic advantages, it is successfully cultivated in rotation with legume grains and small cereals [5]. The small size of C. sativa seed caused an issue in cultivation as seed size directly influenced germination and seedling growth [6]. Camelina seeds are smaller than other oilseed crops, so poor germination and seedling establishment specifically under stressed environments [7]. Different abiotic stress disturbed the physiological and biochemical processes in seeds [8].
Germination or emergence determines the growth and development of plants [9]. The study of these stages is very important for physiological and ecological consequences [10]. It is worth noting that changing climate can affect plant growth and development [11]. This changing environment increases the intensity of environmental stress, which reduces crop production [12]. Water or salt stress, seeding depth, temperature, and pH are the main abiotic factors affecting the germination pattern of plant species [4]. Earlier investigations indicated that seed germination depends on these factors [10, 13, 14]. Temperature is the detrimental factor when all other factors perform ideally, and it plays a role in seed germination by affecting enzyme activity, hormone synthesis, and water imbibition into the seeds [15]. Each species needs a cardinal range of temperature for germination [4, 16]. The suitable temperature at which maximum germination occurs in the shortest duration is desirable for better growth and development [17, 18].
Moisture stress reduces, delays, or prevents the germination percentage or germination rate and eventually affects the seedling growth and development [19]. However, many species overcome drought conditions by producing deep roots if they germinate under water stress conditions [20]. The salinity condition is considered the most harmful abiotic stress, influencing the germination of seeds [21]. Researchers noted that the potential of many species to germinate under salinity makes it possible for future research to explore the salt effects on different stages of plants, starting from germination to seed development. [22]. Soil pH influences the germination and availability of several nutrients [23]. Many plant species require a range of pH for the physiological process. Soil pH was found to determine species distribution by affecting seed germination and seedling establishment [24]. Soil moisture, light, and temperature may vary with the seed depth in the soil, which ultimately determines the germination and emergence of the seed [25]. It was noted that the burial depth of seed and reserve food are interlinked and affect seed emergence [26]. Studies showed that shallow burial of the seed initiates higher germination than surface laying by preventing the seeds and seedlings from drying [27]. The emergence of the seedling is related to the amount of energy present within the seed. A positive correlation is reported between seed mass and emergence ability [28]. Challenges posed by its small seed size: strategies can be employed to optimize germination and seedling growth of C. sativa. These include regulating temperature to match optimal germination range, managing water stress through controlled irrigation, mitigating salt stress with soil amendments or selecting salt-tolerant varieties, and adjusting seeding depth to prevent seed drying and promote germination or emergence. No study has been done on C. sativia seed ecology. Ecological findings of the species will be helpful to determine its potential distribution. It is hypothesized that C. sativa exhibits differential responses in germination and seedling growth under varying environmental conditions. That’s why this study was planned to determine the effect of water and salt stress, pH, temperature, and seeding depth on germination, germination traits, and seedling establishment of C. sativa.
Experimental
Research Location and Source of Seed
The study was carried out in the Department of Agronomy, College of Agriculture, University of Sargodha, Pakistan. Seeds were imported from Canada “Canadian accession” and stored at room temperature (25ºC) in a paper bag until used in the experiment.
Germination Test
Before each experiment, C. sativa seeds were sterilized in sodium hypochlorite 1% for 5 minutes and rinsed 5 times by using distilled water. Twenty-five seeds of C. sativa were placed in a petri-plate with a 9 cm diameter. Each petri-plate was lined with Whatman filter paper No. 10. Treatment solution or distilled water at 3 mL was applied to each petri-plate and was wrapped with Para-film to prevent water loss. The Petri plates were kept in a germinator. The germinator was equipped with bulbs that produced 200 µmol m-2 s-1 PPFD (photosynthetic photon flux density). The bulb was set at a light/dark cycle of 12-h. Each experiment was executed at 25/15ºC day/night temperature, except the temperature experiment. Seeds of C. sativa were considered germinated when the radicle achieved a length of 2 mm. A radicle length of 2 mm was chosen as the germination criterion because it indicates successful initiation of root growth, marking the onset of seedling. The germination was observed daily till no further seed germinated. In the seed burial depth experiment, emergence was considered at the visibility of cotyledon at the soil surface. Each study was repeated two times.
Effect of Temperature on C. Sativa Seeds
The effect of temperature on germination and seedling establishment of C. sativa was investigated at 15/10, 20/15, 25/15, 30/20, and 35/25ºC day/night temperatures. Twenty five seeds of C. sativa were placed on each petri plate and placed in a germinator.
Effect of pH on C. Sativa Seeds
Buffer solutions having pH5 to 10 with an interval of 1 were made to investigate their effect on C. sativa seed germination and establishment. A 2mM solution of MES [2-(N-morpholino) ethane sulfonic acid] was used to prepare a solution of pH 5 or 6, adjusted by 1N HCl. A 2mM solution of HEPES [N-(2-hydroxy-methyl) piperazine-N-(2-ethane sulfonic acid)] was used to prepare a solution of pH 7 or 8, which was adjusted by 1N NaOH. A 2mM TRICINE [N Tris (hydroxymethyl) methylglycine] was used to prepare a solution of pH 9 or 10 and adjusted to each respective pH value with 1N NaOH.
Effect of Osmotic Stress on C. Sativa Seeds
Solutions having osmotic potentials of 0, -0.2, -0.4, -0.6, -0.8, and -1.0 MPa were prepared to investigate their effect on the germination of C. sativa seeds. For the preparation of the solutions, PEG 6000 was used, and the equation of Michel and Kaufmann [29] was used to calculate the known osmotic potential.
Effect of Salt Stress on C. Sativa Seeds
NaCl concentrations from 0 to 300 mM with an interval of 50 mM were prepared to investigate the effect of NaCl concentration on germination, germination traits, and seedling establishment of C. sativa. Solution of each concentration was applied to petri-plate having 25 seeds.
Effect of Seed Burial Depth on C. Sativa Seeds
To investigate the effect of seeding depth on C. sativa, seeds were placed at 0, 1, 2, 3, 4, 5, 6, and 7 in plastic pots with a 15 cm diameter. Each pot was filled with 30, 30, and 40% silt, clay, and sand, respectively. The experiment was kept in a greenhouse at 25±2ºC temperature. Based on the findings of the temperature experiment, this range is conducive to achieving optimal emergence. Adequate moisture was maintained in each pot throughout the experiment. The emergence of seedlings was noted on a daily basis.
Non-linear regression analysis was performed on the germination or emergence data collected in NaCl, osmotic stress, and seeding depth experiments. A 3-parameter logistic model was used for the germination or emergence data of these experiments using Sigma Plot 2008 (version 11.0) software. The fitted model was:
where Gmax= maximum germination, G=germination (%) at x concentration, x50 = NaCl concentration or osmotic potential at which 50% of the maximum germination occurred, and g = slope.
A 3-parameter logistic model:
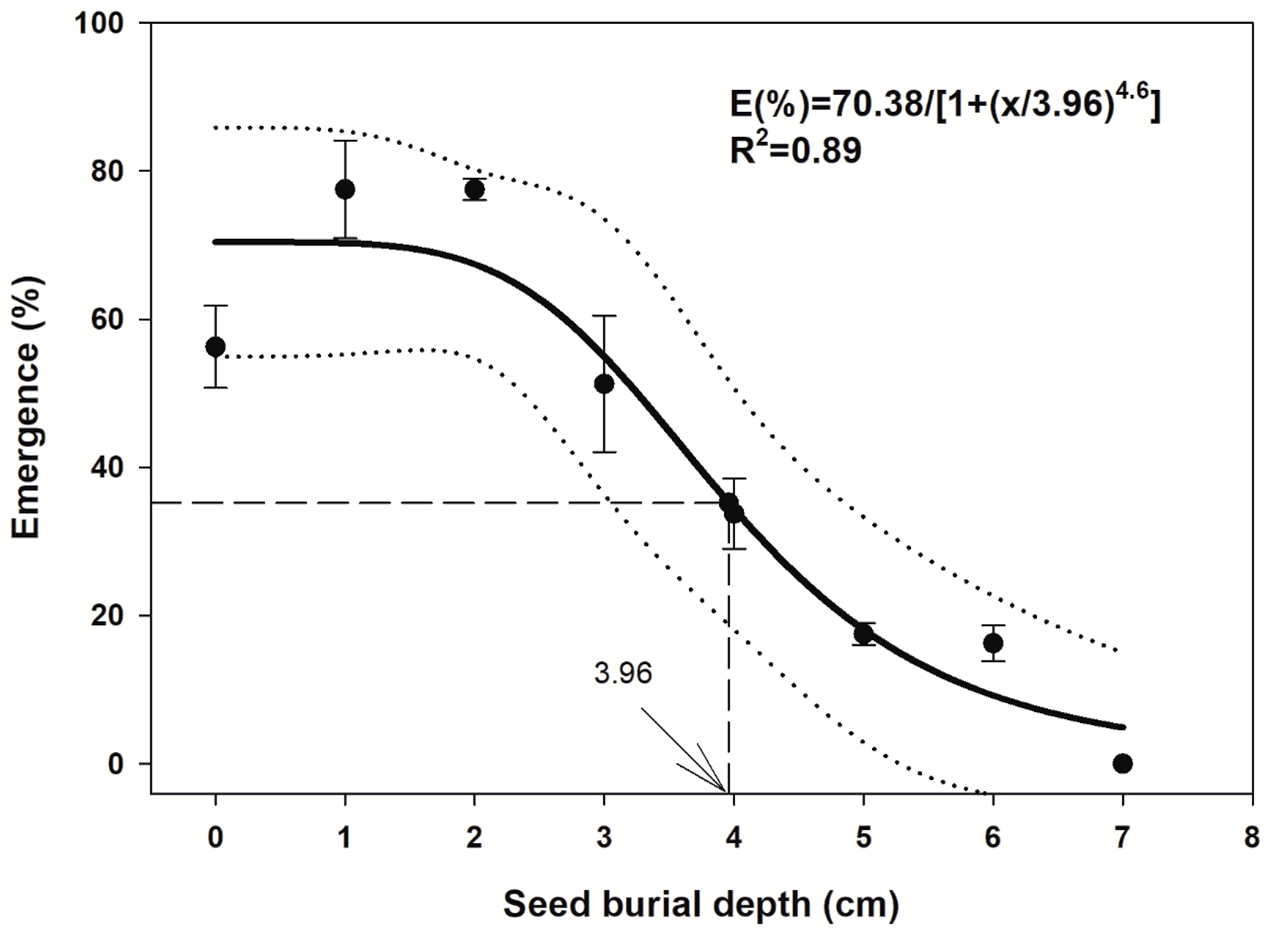
was fitted to data of seeding depth where Emax = maximum emergence, E = emergence (%) at x seeding depth, x50 = seeding depth at which 50% of the maximum emergence occurred, and g = slope.
According to the equation of Coolbear et al. [30].
time taken to 50% germination or emergence was calculated for each experiment.
Where N = final number of germinated or emerged seeds nj and ni = a cumulative number of seeds germinated by adjacent counts are the at times tj and ti, respectively when ni < N/2 < nj.
Mean germination or emergence time (MGTorMET) was calculated according to the equation of Ellis and Roberts [31]:
where Dn = number of germinated seeds on day D and n = number of days start from the beginning.
The equation described by the Association IST [32]:
was used to calculate the germination index (GI) or emergence index (EI). Data regarding the seedling development of C. sativa were collected according to the standard procedures.
Germination parameters such as time to start germination, mean germination time, and germination index are essential for understanding early growth stages and predicting overall crop success. These parameters offer insights into seed vigor, uniformity, and responsiveness to environmental conditions. These parameters, along with germination percentage, help the farmers assess seed quality, anticipate challenges, and optimize planting practices and environmental conditions for uniform seedling emergence and establishment.
Statistical Analysis
Each experiment was performed in a CRD design where each treatment was replicated five times. The data collected were analyzed under the one-way ANOVA technique, and every experiment was repeated twice. The average data of the two repeats is presented. The means were separated with LSD at a 0.05 probability level [33].
Results
Effect of Temperature on C. Sativa
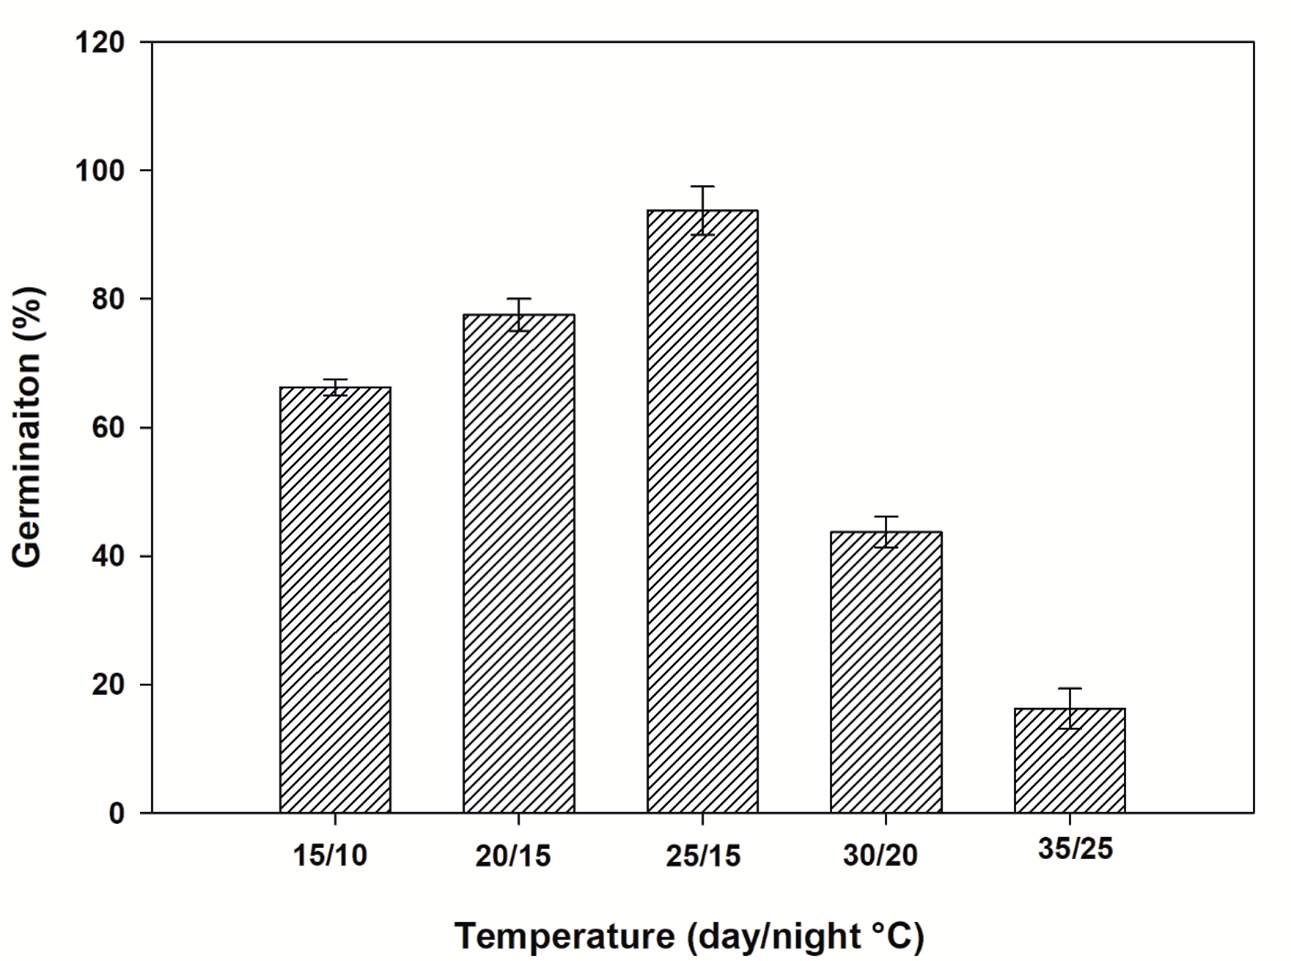
The effect of selected temperatures (15/10, 20/15, 25/15, 30/20, and 35/25ºC day/night) on germination of C. sativa varied significantly (Fig. 1). Maximum germination was counted (93%) at 25/15ºC, considered the optimum temperature for this species. The germination was reduced very quickly when the temperature increased from 25/15 to 35/25ºC. However, 66% germination was observed at the temperature of 15/10ºC. The germination was started 1 day at 20/15ºC as compared to that with 15/10ºC (Table 1). The seeds that were incubated at 35/25ºC took the maximum time to start germination. The minimum T50 and MGT were noted in seeds that were incubated at 25/15ºC and increased when the temperature was increased or decreased to 25/15ºC. The GI was highest (4.13) at 25/15ºC and reduced to 0.43 when the temperature increased to 35/25ºC (Table 1). Among all the temperature ranges, the maximum length of root, shoot, and fresh and dry weight were observed at 25/15ºC (Table 2).
Fig. 1.
Effect of temperature on seed germination of Camelina sativa. Nails on the vertical bars represent standard error of the means.
Effect of pH on C. Sativa
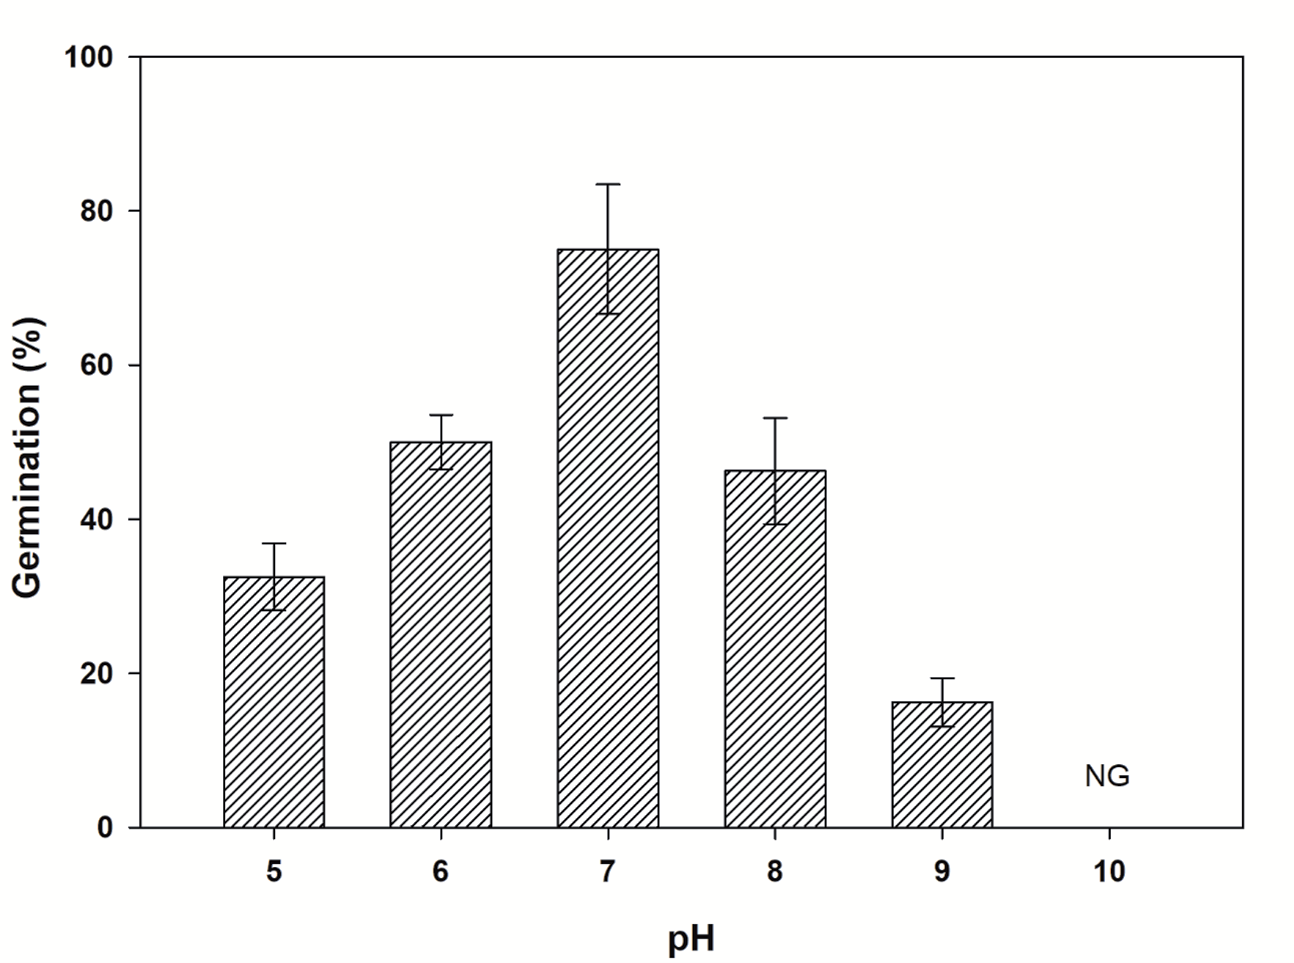
Camelina sativa germination was variable at tested pH levels. Data showed that pH is a limiting factor for germination (Fig. 2). The highest germination (83%) was recorded at a pH level of 7 (control). A steep reduction in germination was noted in an acidic or alkaline medium, where 32% germination at 5 pH and 16% at pH 9 were attained. At a pH level of 10, germination of C. sativa was completely inhibited. Germination of C. sativa was started after 3 days of sowing with distilled water or a pH level of 7 (Table 1). Alkaline medium delayed the germination up to 4 days compared to that of the control treatment or pH level of 7. However, an acidic medium (pH 5) delayed the germination for 1 day when compared to the control treatment. Similarly, T50 and MGT were the lowest at a pH level of 7 and increased with an increase or decrease in pH level from 7. The GI was highest at pH level 7, while it reduced at a higher rate with an alkaline medium than that with an acidic medium. Seedling development of C. sativa was highest at pH 7 (Table 2).
Effect of Osmotic Stress on C. Sativa
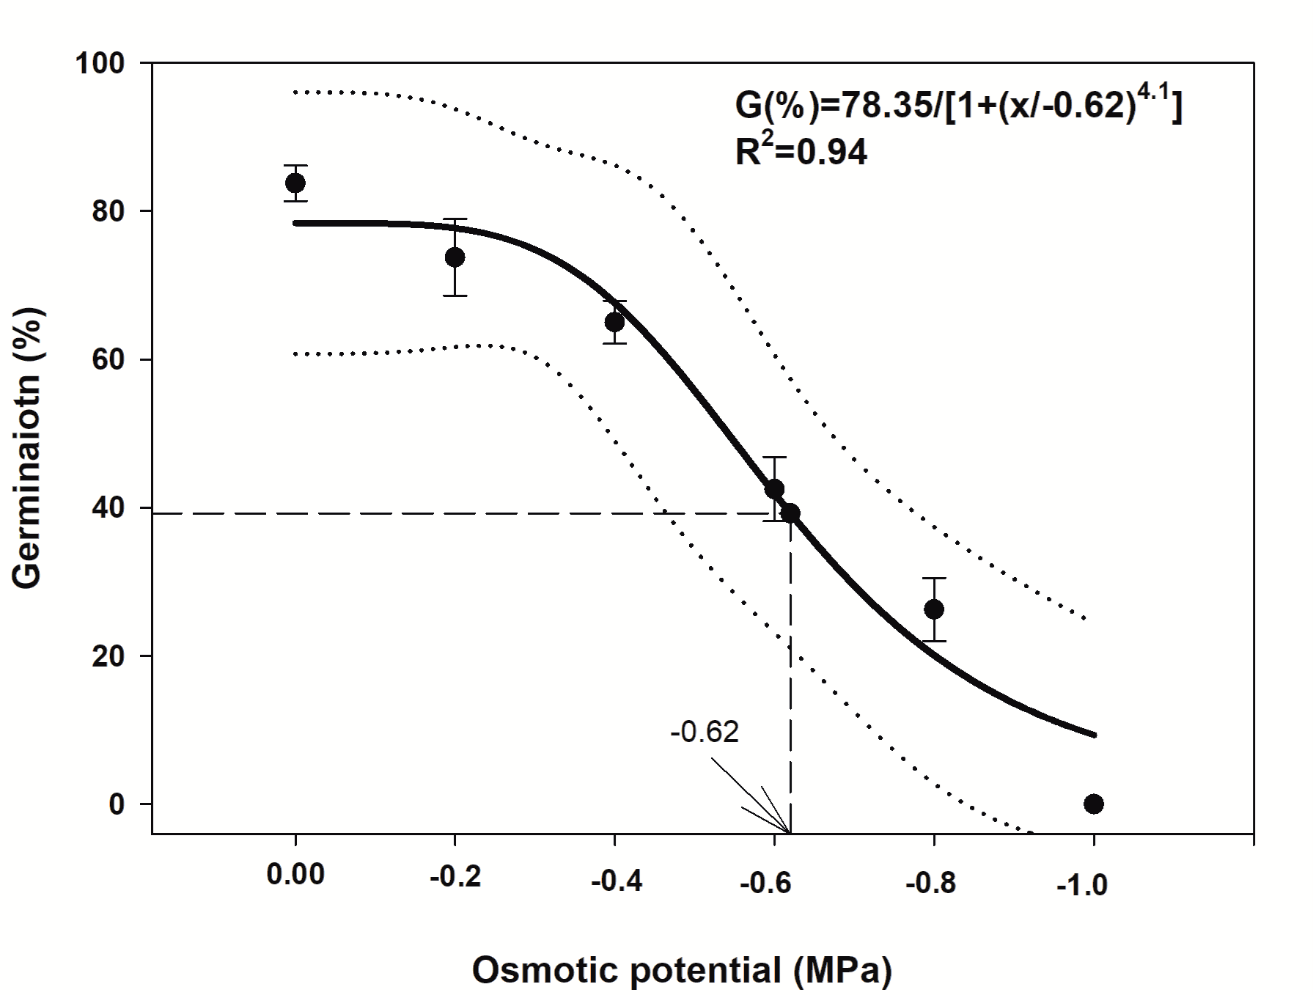
The logistic model with three parameters was used to evaluate the germination percentage of C. sativa under tested osmotic potentials (Fig. 3). The model estimated that germination of C. sativa decreased from 83 to 26% when osmotic potential decreased from 0 to -0.8 MPa. The germination was completely inhibited when the osmotic potential was approached to -0.1 MPa, and the model predicted 50% germination at 0.62 MPa. Different osmotic potentials showed a significant difference in time to start germination. C. sativa seeds started germination within 4 days when the seeds were incubated at -0.2, -0.4, or control treatment. After that, germination was delayed with an increase in osmotic potential and delayed up to 7 days with -0.8 MPa osmotic potential. Likewise, T50 and MGT were increased with -0.6 or -0.8 MPa osmotic potential when compared to higher osmotic potential or control treatment (Table 1). Camelina sativa seed showed similar GI at -0.2 to -0.4 MPa osmotic potentials and control treatment, while at -0.8 MPa osmotic potential GI decreased to 0.56. Root length was significantly reduced with -0.8 MPa osmotic potential when compared to other osmotic potentials (Table 2). However, the control treatment measured the maximum length of C. sativa roots. A decline in shoot length from 3.61 to 2.48 cm was noted when potential was reduced from 0 to -0.8 MPa. Camelina sativa seedlings could tolerate the moisture stress and reduced the fresh and dry weight with deceased in osmotic potential even at -0.2 MPa, and dry weight was reduced to 50% with the lowest osmotic potential (-0.8 MPa) when compared to the control treatment (Table 2).
Table 1.
Effect of environmental factors on time to start germination or emergence, time taken to 50% germination or emergence, mean germination or emergence time and germination or emergence index of Camelina sativa.
[i] Note: The values sharing the same letters did not differ significantly at P≤0.05. T50 or E50, time taken to 50% germination or emergence; MGT or MET, mean germination or emergence time; GI, germination index; EI, emergence index; NG or NE, no germination or emergence; SE, standard error. Values in the parentheses are standard errors of the mean.
Table 2.
Effect of environmental factors on shoot and root length (cm) and fresh and dry (g per plant) of Camilena sativa.
Effect of Salt Stress on C. Sativa
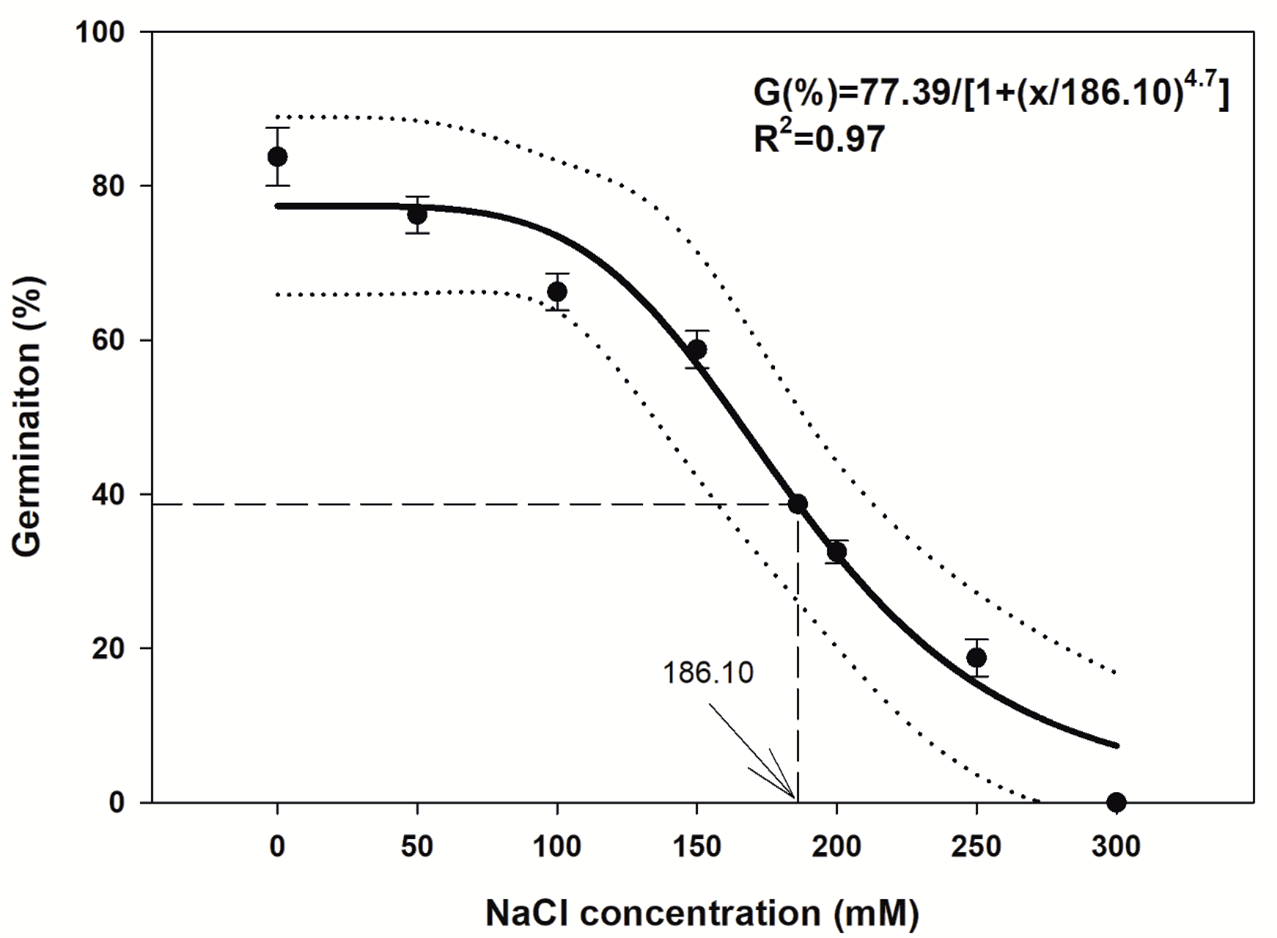
A logistic model with three parameters was used to estimate the effect of different NaCl concentrations on the germination of C. sativa. (Fig. 4). The model estimated that NaCl 100 to 250 NaCl concentration reduced the seed germination linearly. Given that only 18% of seeds were germinated at a concentration of 250 mM, however, similar germination was recorded at 50 mM or control treatment. The concentration of 300 mM completely inhibited the germination of C. sativa. According to the fitted model, 50% germination of the maximum has occurred at 186 mM. Germination start time was increased with an increasing salt concentration, and germination was delayed for 1 day and 5 days at 100 and 250 mM, respectively (Table 1). The MGT or T50 was bottommost in control compared to other tested concentrations. In contrast, the control treatment recorded maximum GI. Seedling establishment, such as biomass production and root and shoot length, were significantly reduced compared to that with distilled water (Table 2).
Effect of Seeding Depth on C. Sativa
The logistic model was fitted to estimate the response of C. sativa seed to varying seeding depths (Fig. 5). Seeds sown on the soil surface recorded 56% germination, while the emergence percentage of C. sativa seeds was 77% when placed at 1 or 2 cm of soil depth. After that, the emergence was reduced linearly and recorded only 16% emergence when the sowing depth was 6 cm. Seedling emergence of C. sativa was completely inhibited at 7 cm depth. According to the fitted model, 50% of the maximum emergence would have occurred at a seeding depth of 4 cm. Emergence times (start time, E50, MGT) were linearly proportional to seed burial depth (Table 1). Seeds that were buried at 1 or 2 cm emerged earlier than seeds placed at a depth of 4 or 5 cm. Moreover, the time to start germination is delayed in the seeds placed on the soil surface. The E50 and MET were minimum, and the EI was maximum when seeds were placed at 1 cm. Root and shoot lengths of C. sativa seed at the depths of 0-3 cm were similar to each other; after that, the lengths were reduced. The fresh weight of C. sativa plants was minimum under the seed burial depth of 6 cm (Table 2).
Discussion
Germination is affected by ecological conditions prevailing in the habitat. Germination responses for C. sativa to various environmental factors were tested to identify the possible planting windows appropriate for this species. It depends on light, temperature, moisture, and abiotic stress. Among the factors, temperature plays a key role in the germination, growth, and development of plants, as its mechanism of action is quite complex [4, 26]. Temperature influences each step of germination in different ways. The critical temperature of seed germination is different for each species. According to Russo et al. [34], temperature influenced the germination time of mustard and camelina, and this variation was notable within varieties. Data from this experiment showed that the suitable temperature for this species is 25/15ºC. A previous study showed that C. sativa showed maximum germination (100%) between 16 and 27ºC, while germination reduced to 80% when the temperature increased to 32%ºC [34]. Germination parameters, especially time parameters, were ideal at 25/17ºC and increased with an increase in temperature, indicating that this species will not grow successfully if exposed to other climates. Root and shoot development were highest at 25/15ºC, as verified by the results of Benvenuti et al. [35], who found that temperature beyond the optimum level was detrimental to growth and development. According to Mobli et al. [36] root and shoot dry weight were affected by little increase or decrease from the optimum temperature in many plant species.
Our findings showed that the germination of C. sativa was influenced by pH ranges. A quick decline in germination was noted in acidic or alkaline medium, and there was no germination of seed pH 10. Many plant species may germinate over a wide pH range, but some species showed difficulty in germination when exposed to extreme alkaline conditions [17]. T50 and MGT were increased in an alkaline medium, which might be due to the increased concentration of salt. A study by Deska et al. [37] proved a negative effect of growing medium acidity on germination and seedling establishment of Trifolium repens and Medicago sativa. Unfavorable conditions at the initial germination stage of C. sativa affected the germination parameters (time to start germination, T50, MGT, and GI), which led to weaker development of plant seedlings. Previous studies depicted that lower or higher pH levels influenced nutrient absorption by roots during seedling growth.
Water required for seed germination depends on seed size and species. Given that dry seeds required more water quantity for imbibition and other germination processes. Germination of C. sativa was reduced with the reduction in osmotic potentials, and no germination was recorded when the seeds were subjected to -1.0 MPa osmotic potential. The process of water imbibition varied in different seeds depending on their sensitivity to drought conditions. Seeds of Russian knapweed and perennial pepper were exposed to 0.0, -0.2, -0.4, and -0.6 MPa osmotic potentials, and results showed that Russian knapweed was more sensitive to the osmotic potential as compared to perennial pepper weed [38]. Different osmotic potentials resulted in variable germination parameters over time. The time to start germination was delayed up to 7 days under the maximum water stress condition. The reduction in seed and seedling traits in water stress conditions might be due to osmotic stress and disturbance in the cell physiology of the plants that inhibit water absorption. It is documented that enzyme activity is suppressed by severe water stress, which ultimately reduces carbohydrate metabolism and reduces the water potential. Moreover, water stress reduced the calcium and potassium uptake and changed the seed hormones in the germination phases [39]. Our results showed that water stress reduced root, shoot length, and weight. Under water stress conditions, enzyme activity is disturbed, which leads to altering the hydration status of cells and disrupting biochemical reactions. Enzymes that involve breaking down stored nutrients in the seed to provide energy for germination might be affected under these stress conditions. Moreover, moisture stress causes the accumulation of reactive oxygen species within cells, which can damage enzymes and other cellular components. Less availability of water reduced the development of root and shoot, which supported the findings of Białecka and Kępczyński [40], who found that water availability played a critical role in enzyme activity in the hydrolytic breakdown of carbohydrates, lipids, proteins, and transportation of metabolites in the germinating seeds. Moreover, the amylase enzyme is activated during imbibition, which converts endosperm starch into metabolizable sugar and supplies the energy for the root and shoot growth of seedlings [40].
Many plant species are sensitive to salinity, and their germination is negatively affected under saline conditions [36]. However, some species are tolerant to salinity and may successfully germinate under such conditions [38]. Our results indicated that C. sativa germinated well under slight saline conditions, but germination reduced to 18% at 250 Mm NaCl concentration. It is documented that higher salt concentrations inhibited the germination of many plant species, and plants may die at any developmental stage, whereas some species are tolerant of salinity conditions. Salt stress interferes with enzyme activity, similar to water stress. Salt ions can directly inhibit the activity of certain enzymes or disrupt their structure, impairing biochemical reactions necessary for seed germination and growth. Furthermore, salt stress induces oxidative stress in plants, leading to the production of ROS and causing damage to proteins, lipids, and nucleic acids. Two mechanisms are reported through which salinity reduces germination and growth: salinity may create difficulty in moisture uptake or intake of toxic ions, which disrupt the hormonal and enzymatic action during germination and growth. Gupta and Penday [41] reported the inhibition of germination in Phaseolus vulgaris was due to the osmotic effect of NaCl with increasing concentration. Further, the salt stress reduces the entry of water or facilitates the absorption of toxic ions, which leads to hormonal imbalance and results in the inhibition of germination. Salinity might affect some physiological processes in plants, but it is unclear whether the reduction in germination is directly due to osmotic effects or to some non-toxic germination repression caused by the salt. Under osmotic stress conditions, the PEG is either unable to cross the cell membrane or can do so only slowly, while in the case of salt stress, salt might be compartmentalized and the seed avoids the negative effect of low water potential. Kim and Park [42] supported the second mechanism and reported inhibition of the biosynthesis of gibberellin under salinity conditions, which is a hormone used in seed dormancy and growth. Moreover, salt stress disrupts physiological and chemical processes in seeds and plants.
Seeding depth is considered a critical factor in the evaluation of seed size, seed emergence, and survival of the seedling and young plants. Moreover, germination is directly related to the seeding depth. C. sativa seeds that were planted on the surface of the soil showed less germination than the seed placed at 1 or 2 cm. However, emergence was reduced linearly with an increase in depth, and seeds completely failed to emerge when the burial depth was 7 cm. Our findings are in agreement with the findings of Ren et al. [27], who depicted that seeds buried in shallow soil showed more germination than the seeds planted at the soil surface because it kept the environment moist around seeds and prevented drying out of seeds and seedlings. Excessive burial of seeds affected the seed germination and emergence. In contrast, bulky-sized seeds have additional food reserves and can appear from deeper depths [43]. Our results depicted that seeds of C. sativa placed at a deeper depth required more time for emergence. Seeds of the dove weed placed at 2 cm to 6 cm needed more time to emerge and complete 50% germination in 3 more days when compared to that placed on the soil surface [44, 45]. Root and shoot development of C. sativa decreased with an increase in seeding depth. These findings are further supported by [22], who documented that increased burial depth of some species, and root and shoot growth decreased significantly.
It is concluded from the study that there is a strong relationship between environmental factors and the germination attributes of C. sativa. Optimum germination and seedling growth occur at 25/15ºC day/night, with sensitivity observed towards extreme temperatures. Osmotic potential and seeding depth also significantly influence germination and emergence, with complete inhibition noted under certain conditions. These findings showed the importance of understanding seed ecological factors for determining suitable cultivation localities and potential distribution in new environments, particularly in problematic soils. By integrating this knowledge into cultivation strategies, farmers can mitigate risks and enhance the efficiency and sustainability of C. sativa production, ultimately contributing to its potential as an alternate low-input oilseed crop.

