


Introduction
Insecticides are increasingly used in fruit production to control harmful insects and to increase fruit yield and quality. Peach moth (Grapholita molesta Busck) is an economically significant pest of stone and apple fruits worldwide, including in the Republic of Serbia. Due to the incorrect and delayed application of insecticides, the caterpillars of the peach moth primarily infest the offshoot branches and subsequently the fruit, leading to a reduction in both the yield and quality of the peach fruit. On the other hand, their inappropriate and intensive application can lead to harmful effects on cultivated plants, causing disruptions in physiological and enzymatic processes that ultimately impact overall yield and result in the presence of pesticide residues [1]. Insecticides affect plants through various mechanisms, including inhibition of biological processes such as photosynthesis. Another consequence of unsuitable pesticide application is phytotoxicity, which is reflected in changes in the form of chlorosis and necrosis of leaves that lead to the complete decay of plant tissue. Physiological, biochemical, and genetic characteristics of plants influence the accumulation of chlorophyll and carotenoids [2]. The content of photosynthetic pigments in plants is an important indicator for the determination of photosynthesis productivity [3]. Stress can either inhibit the synthesis or enhance the degradation of photosynthetic pigments, changing the photosynthetic activity of plants and the production of organic matter [4]. The application of some pesticides can reduce the content of photosynthetic pigments in plants [5]. Carotenoids also play an important role in increasing the use of light in photosynthetic systems, i.e., increasing absorption efficiency. They also have antioxidant properties, and therefore they are important in the protection of chlorophyll from the harmful effects of extreme light intensity that can cause their photooxidation and destruction.
It has been proven that some insecticides (organophosphates, carbamates, and pyrethroids) negatively affect photosynthesis [6]. Organisms that use oxygen for their growth and development face the highly reactive process of oxygen derivatives. Free radicals are atoms, molecules, ions, or even groups of atoms or molecules with one or more unpaired electrons in an orbital. However, reactive oxygens also include components without unpaired electrons in the orbital (so-called reactive nonradical agents), such as hydrogen peroxide (H2O2) [7]. Low and moderate concentrations of these substances are typically present during cellular metabolic activity and play important roles in various reactions. High levels of free radicals induce oxidative stress, which serves as a precursor to numerous pathological conditions. Free radicals are produced in the plant cell by the aerobic metabolism process, as intermediate products of the oxidation of water to molecular oxygen in the photosynthetic electron transport chain [8]. The occurrence of oxidative stress in plants can be caused by various abiotic factors - drought, increase in salinity, increased or decreased temperature, heavy metals, and other pollutants. Plants possess a highly efficient system of antioxidant enzymes, including superoxide dismutase (SOD), ascorbate peroxidase (APX), pyrogallol peroxidase (PPX), and catalase (CAT), which control the production of ROS and protect plant cells, reducing the level of oxidative stress [9]. The cell membrane is composed of unsaturated fatty acids. During oxidative stress, membranes become vulnerable to free radicals, leading to lipid peroxidation that changes their selectivity and disrupts cellular physiological functions [10]. The damage caused by lipid peroxidation is monitored by measuring the amount of some of the final products. Typically, the amount of malondialdehyde (MDA), 4-hydroxynonenal (HNE), and isoprostane is measured. Malondialdehyde is detected through the reaction with thiobarbituric acid (TBA), forming colored products of thiobarbituric reactive substances (TBARS). Lipid peroxidation and malondialdehyde affect cell membrane, ion transport, and phospholipid exchange between two lipid layers. They also reduce membrane fluidity but increase membrane permeability for some substances that could not pass through the membrane before oxidative stress [11]. Numerous studies confirmed the influence of pesticides on different processes in plants; however, there is still a lack of data when it comes to peaches and insecticides used in pest management. In our previous study, conducted in 2019, at the localities Šišatovac and Čelarevo, the adverse impact of insecticides on the total chlorophyll and carotenoids in peach leaves has been shown [12]. However, this research aimed to evaluate the influence of the mainly applied insecticides for the control of G. molesta on physiological and biochemical processes in peach leaves through total chlorophyll, carotenoids, as well as hydrogen-peroxide and malondialdehyde as oxidative stress parameters. The trial was carried out in an area with intensive peach production.
Material and Methods
The determination of the chlorophyll and carotenoid content in the peach leaf was carried out during 2020 in the Plant Physiology Laboratory (Department of Crop and Vegetable Production, Faculty of Agriculture, Novi Sad, Serbia). Besides, the influence of insecticides on H2O2 and MDA as well as on the fresh and dry weight of peach leaves was analyzed. Insecticides used in the experiment are shown in Table 1. The experiment was set up in peach orchards (“Royal Gem” variety) at the locality of Mala Remeta (Republic of Serbia) in three replications for each insecticide, including the untreated control. Insecticides were applied foliarly with water consumption of 1000 L/ha during the BBCH 75 phenophase of the peach. For the laboratory analysis, the youngest fully developed peach leaves were sampled three and seven days after the treatment on the sun-exposed side of the orchard (three top leaves per tree). The extraction of chlorophyll a, b, and carotenoids from fresh leaves was performed with acetone.
Table 1.
Applied insecticides.
Fresh leaves are cut, and 0.2 g is macerated with 10 mL of 100% acetone. The extract is filtered with the addition of acetone to a final volume of 25 mL and analyzed. Absorbances were measured at wavelengths of 440, 644, and 662 nm on a Shimadzu UV-VIS-1240 spectrophotometer. For the calculation of the concentration of the pigments in acetone extracts, molar absorption coefficients according to Holm and Von Wettstein were used. The concentration of hydrogen peroxide (H2O2) was determined according to the method of Alexieva et al. [13]. For the analysis, plant material (0.5 g) was homogenized using liquid nitrogen and extracted with 5 mL of 0.1% trichloroacetic acid (TCA) and centrifuged. Afterward, the supernatant was separated (0.5 mL) and mixed with 0.5 mL of 10 mM potassium phosphate buffer (pH 7.0) and 2 mL of reagent (1 M KI). As a blank, 0.5 mL of 0.1% TCA is used. The absorbance was also measured spectrophotometrically at 390 nm wavelength. The intensity of lipid peroxidation was determined from the malondialdehyde (MDA) extracted from fresh plant material (peach leaves) using a mixture of thiobarbiturate (TBA) and TCA and perchloric acid (PCA) in a ratio of volume 1:3. The concentration of pigments in the leaves was calculated and expressed in mg/g of fresh mass of peach leaves. The fresh mass was measured at the beginning of the analysis, immediately after sampling, while the content of dry matter was determined by drying the samples to a constant mass at a temperature of 70°C. The obtained data were statistically analyzed using ANOVA and LSD tests for a confidence interval of 95% in the statistical program R ver. 3.2.2.
Results and Discussion
Determination of Chlorophyll and Carotenoid Content in Peach Leaves
In Tables 2 and 3 and Fig. 1, results of the effect of applied insecticides on the content of chlorophyll and carotenoids in peach leaves are shown. The obtained results indicate a reduction in the content of chlorophyll (a+b) from 6.94 to 43.06% in all samples, three days after the insecticide application. The carotenoid content was reduced (1.96%) after the treatment with chlorantraniliprole (0.50 mg/g) and acetamiprid (0.50 mg/g), while in the leaves from the other treatments, carotenoid content increased from 3.92% to 27.45%, compared to the untreated control (0.51 mg/g). The application of cyantraniliprole (0.51 mg/g) did not cause a change in the concentration of the pigments (Table 2). However, all applied insecticides (except deltamethrin) affected a significant decrease in the content of chlorophyll (a+b) (F = 54.03; p<0.01**; LSD = 0.18), while pyriproxyfen significantly increased carotenoids by 27.45% (F = 21.56; p<0.01**; LSD = 0.09).
Table 2.
Concentration of pigments in the leaf (mg/g) three days after insecticide application.
Table 3.
Concentration of pigments in the leaf (mg/g) seven days after insecticide application.
Fig. 1.
Concentration of pigments in the leaf (mg/g) three and seven days after insecticide application.
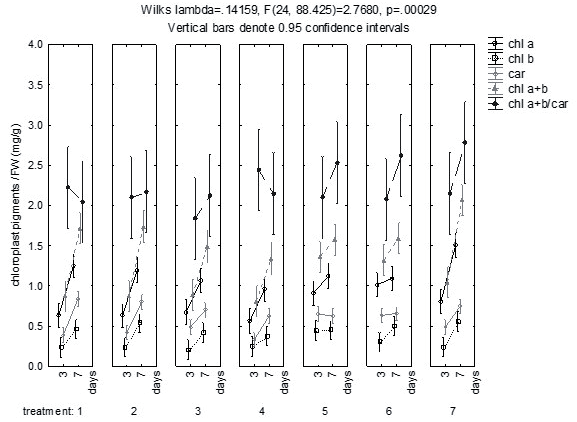
Seven days after the treatment, chlorophyll (a+b) content decreased from 7.35% to 38.37% (Table 3). The content of carotenoids decreased in the treatments with pyriproxyfen (0.43 mg/g), deltamethrin (0.46 mg/g), and acetamiprid (0.60 mg/g) from 3.23% to 30.65%, while the other treatments influenced an increase from 3.23% to 41.94%, i.e., 0.64-0.88 mg/g.
Seven days after the treatment, statistically significant differences were recorded (F = 229.69; p<0.01**; LSD = 0.15) in the content of chlorophyll (a+b) in the peach leaves treated with insecticides and the control. The content of carotenoids significantly increased in the treatment with cyantraniliprole and spinetoram, while it decreased in the treatment with deltamethrin and pyriproxyfen seven days after the application (F = 143.25; p<0.01**; LSD = 0.11). Significant differences after the application of chlorantraniliprole and acetamiprid were not recorded.
Based on the ratio of concentrations of total chlorophyll (a+b) and carotenoids (Fig. 1), it can be stated that the obtained values are at approximately the same level compared to the control variant, three and seven days after the application of insecticides.
Analysis of Hydrogen-Peroxide and Malondialdehyde Content in Peach Leaves
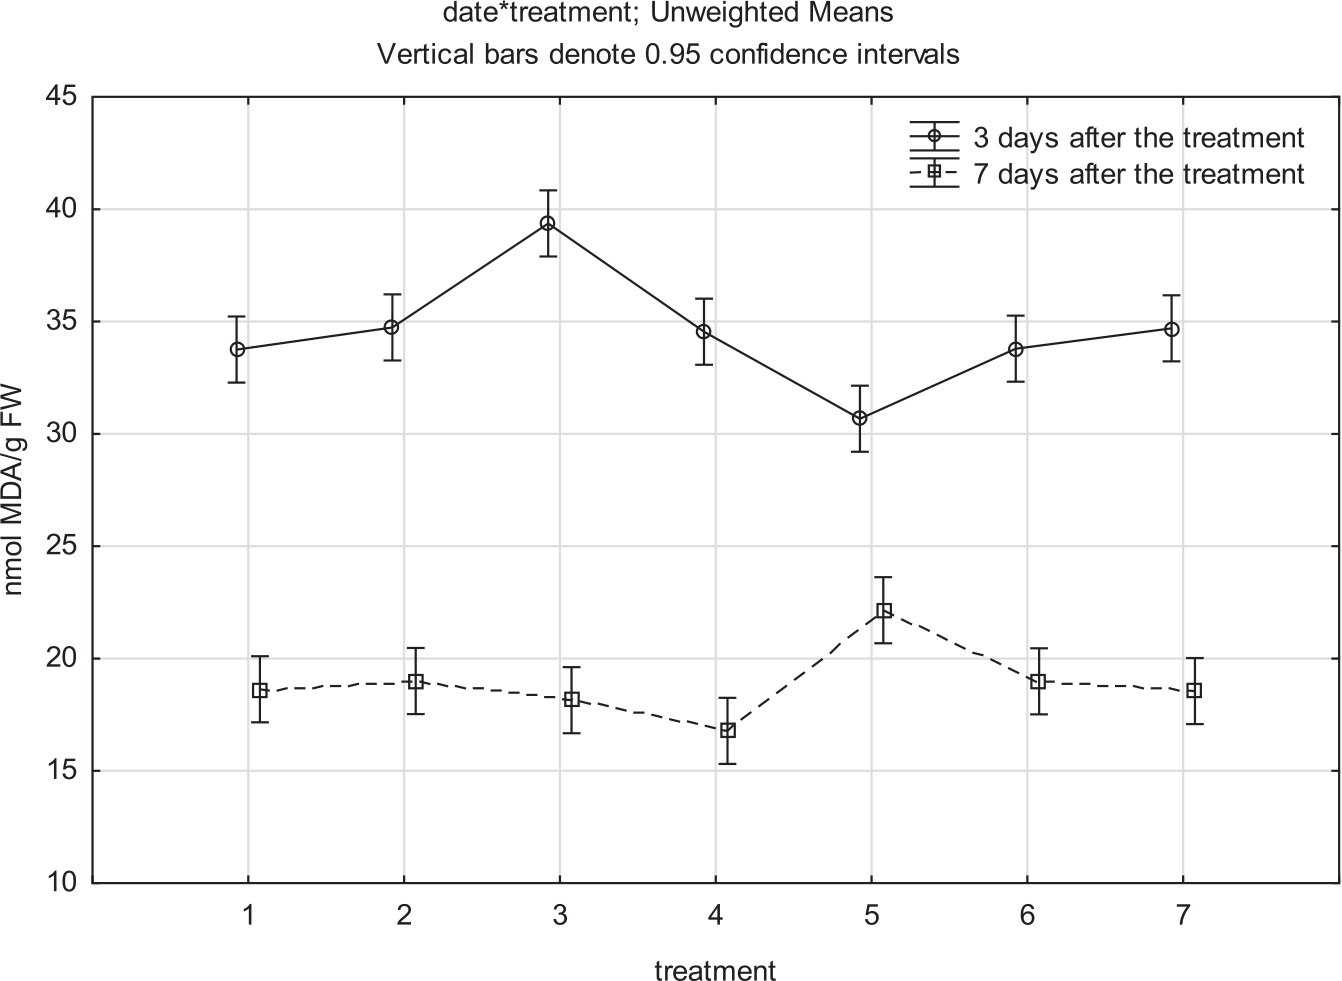
Three and seven days after treatment, the concentrations of hydrogen peroxide (H2O2) and malondialdehyde (MDA) in peach leaves were analyzed (Fig. 2 and 3). Three days after the treatment, there were no significant differences between the treatments and the control, while after seven days, the concentration of H2O2 increased (30 to 80%) (30-45.2 µmol/g fresh weight (FW)). The highest increase in H2O2 concentration was found after deltamethrin and spinetoram application (50-85%). The results of the analysis of MDA (an indicator of the degree of lipid peroxidation) three and seven days after exposure to insecticide are shown in Fig. 3. The concentration of malondialdehyde in all samples was higher three days after treatment (31-39.3 nmol/g FW) concerning the concentration of MDA in the samples after seven days, including the control (30-22.5 nmol/g FW). The difference in malondialdehyde concentration seven days after treatment was generally smaller than after three days. Three days after the treatment, the concentration of MDA was higher compared to the control. At the locality of Mala Remeta, an increase in the concentration of MDA was recorded in samples treated with chlorantraniliprole (13%), while in those treated with deltamethrin, the concentration decreased (11%), compared to the control. Seven days after insecticide application, MDA concentrations were at the same level as the control variant, except for deltamethrin, where MDA concentration increased (19%) and acetamiprid with decreased MDA (10%) was recorded.
Determination of Leaf Fresh Weight and Dry Matter Content
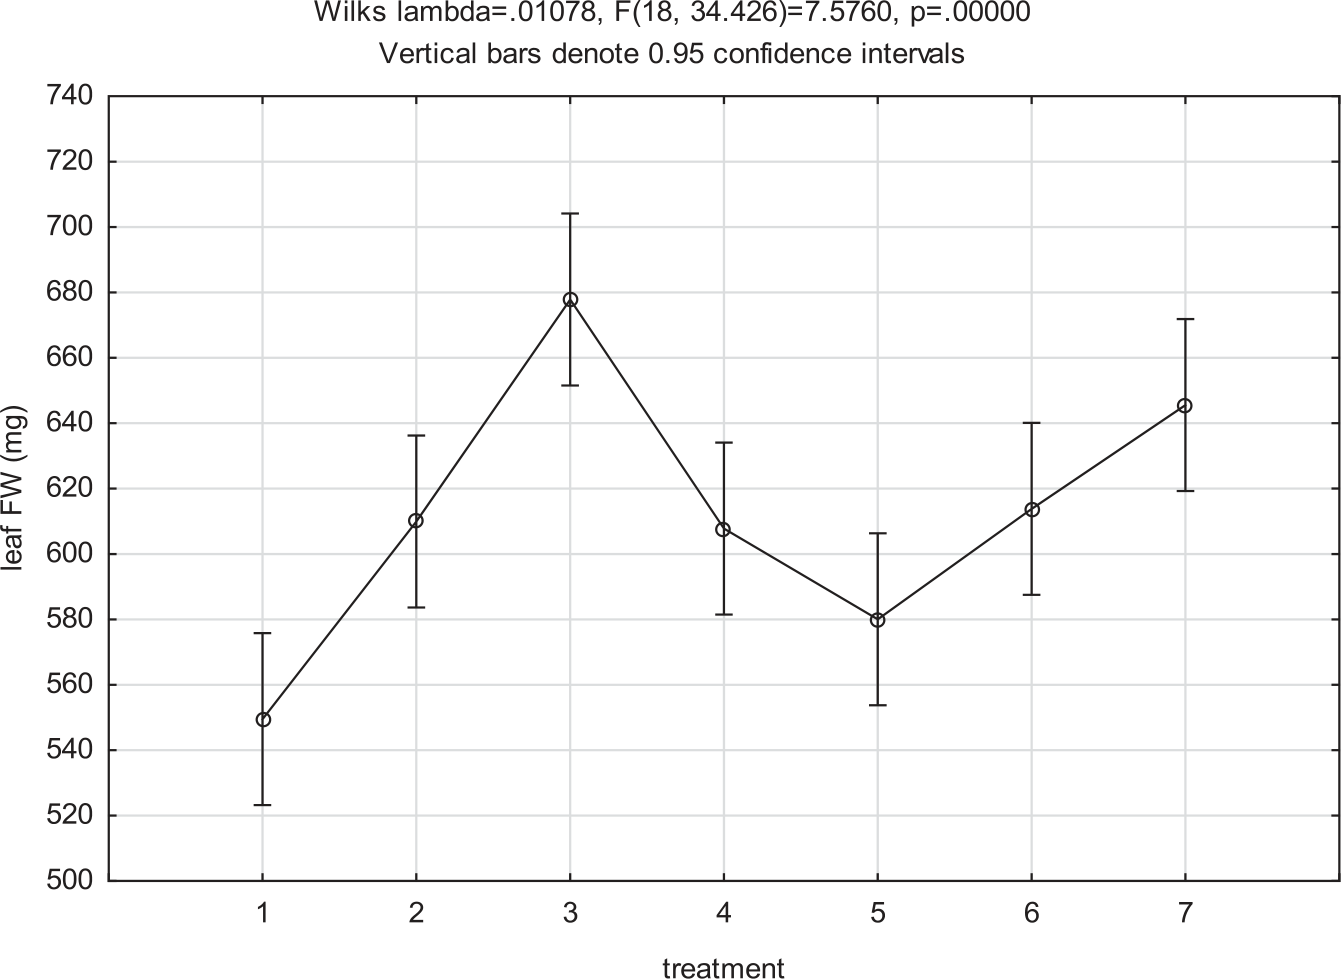
The results of the effect of applied insecticides on the fresh and dry leaf masses are shown in Fig. 4 and 5. A slight increase in the fresh and dry leaf mass (9%) was found after the treatment with chlorantraniliprole, while the lowest value was obtained in the treatments with cyantraniliprole and deltamethrin, with a decrease of 10-22% in both fresh and dry weight of peach leaves.
Fig. 2.
Concentration of H2O2 (µmol/g FW). (1: cyantraniliprole; 2: spinetoram; 3: chlorantraniliprole; 4: acetamiprid; 5: deltamethrin; 6: pyriproxyfen; 7: control).
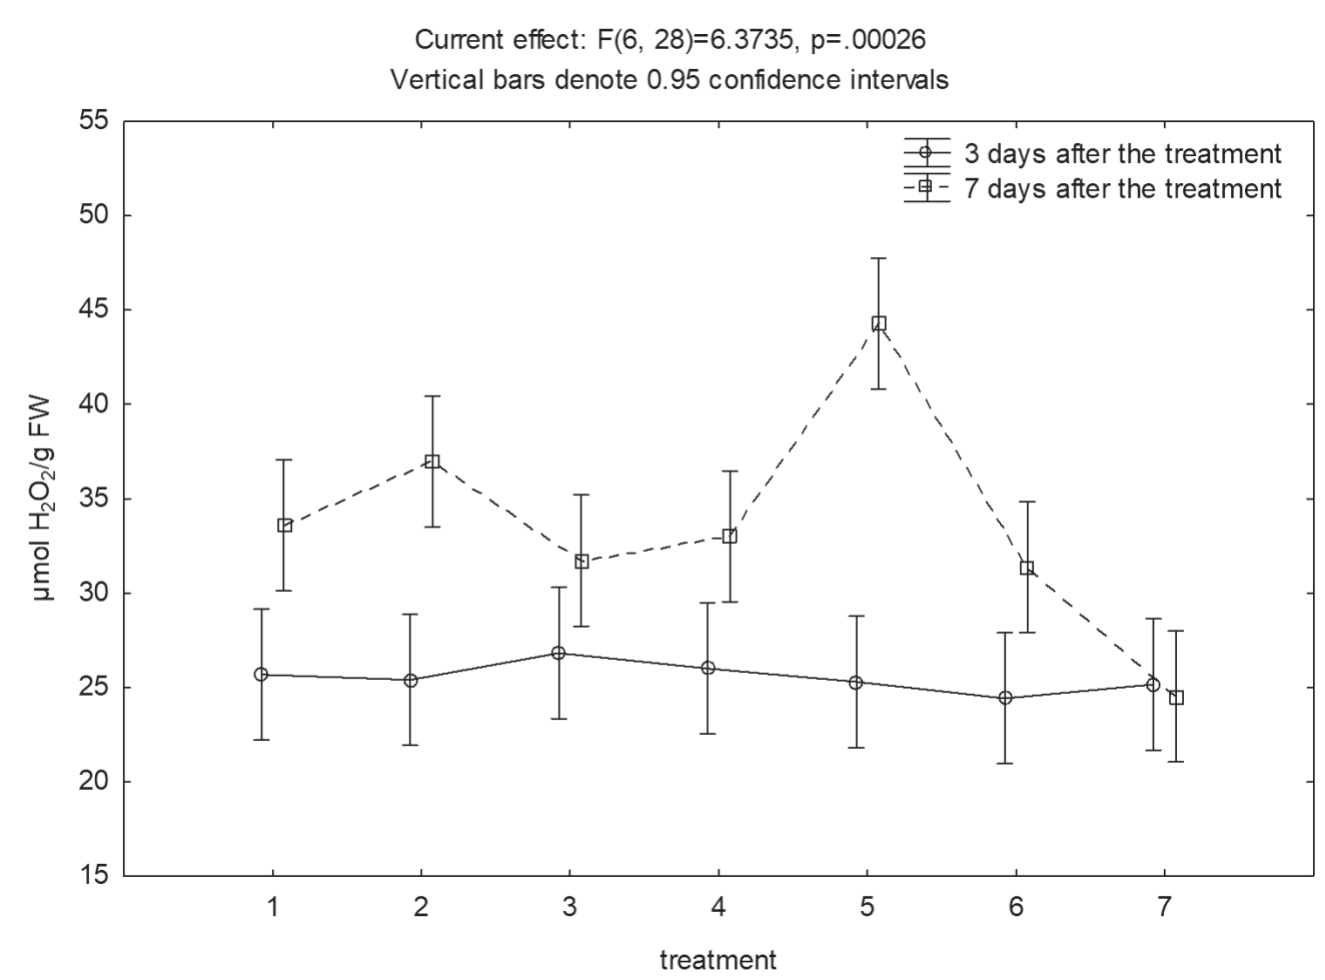
Fig. 3.
Concentration of MDA (nmol/g FW). (1: cyantraniliprole; 2: spinetoram; 3: chlorantraniliprole; 4: acetamiprid; 5: deltamethrin; 6: pyriproxyfen; 7: control).
Inhibition of photosynthetic pigments due to the application of pesticides can reduce photosynthetic activity in plants [5]. Application of pesticides can affect young plants, leading to an alteration in biochemical, physiological, and different enzymatic and non-enzymatic processes [14]. Also, pesticide application causes oxidative stress in plants through reactive oxygen species [15]. This ultimately leads to a decrease in the growth and photosynthetic activity of plants. Different insecticide groups (organophosphates, carbamates, and pyrethroids) cause diverse effects of photosynthesis [6]. In this study, applied insecticides led to changes in the concentration of chlorophyll and carotenoids in peach leaves. They mainly affected the reduction of total chlorophyll content in leaves three and seven days after treatment, while the content of carotenoids increased in almost all samples three and seven days after treatment, except after the application of spinetoram and chlorantraniliprole.
Fig. 4.
Fresh leaf mass (mg). 1: cyantraniliprole; 2: spinetoram; 3: chlorantraniliprole; 4: acetamiprid; 5: deltamethrin; 6: pyriproxyfen; 7: control).
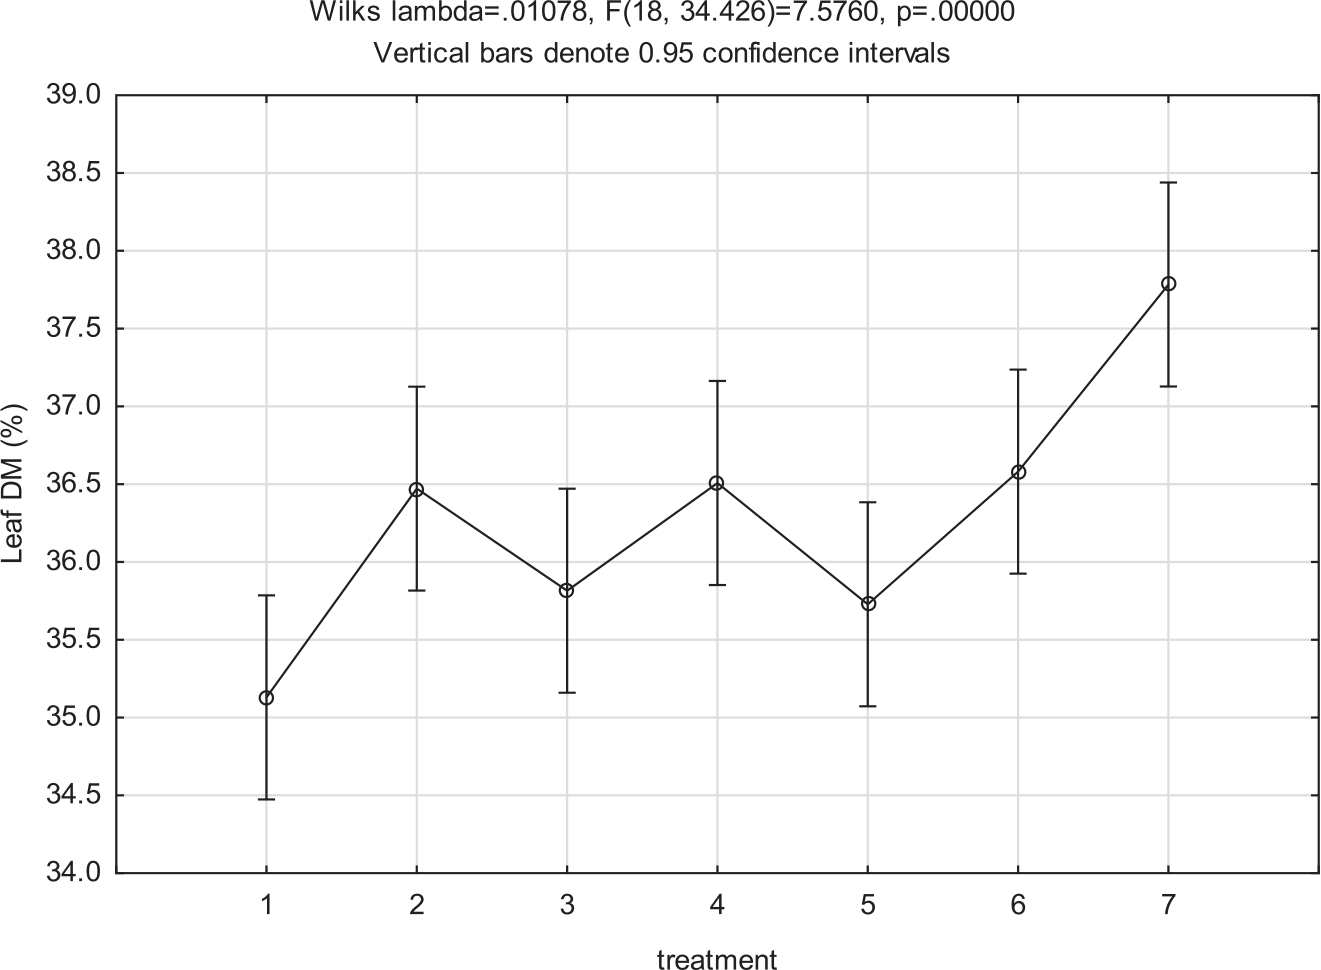
Fig. 5.
Dry leaf mass (%). (1: cyantraniliprole; 2: spinetoram; 3: chlorantraniliprole; 4: acetamiprid; 5: deltamethrin; 6: pyriproxyfen; 7: control).
Opposite to these results, after the application of the insecticide spinetoram, tomato plants were significantly superior, which was confirmed by the high chlorophyll [16]. Moreover, the application of chlorantraniliprole (30.2%), indoxacarb (13.1%), and their mixture (26.8%) increased the content of chlorophyll a and b in tomato leaves [17], confirming the results obtained for chlorophyll a. Based on the studies of the influence of deltamethrin on the biological characteristics of maize obtained results showed a decrease in pigment content as the concentration of deltamethrin increased (chlorophyll a by 7-87% and chlorophyll b by 6-52%, carotenoids by 8-76%) [18]. Also, it is concluded that the content of photosynthetic pigments in maize was significantly lower in treatments with chlorantraniliprole compared to the control. The content of chlorophyll a, b, and carotenoids decreased by 70%, 63%, and 65%, respectively. Furthermore, in this study, chlorophyll (a+b) in peach leaves was reduced by 6.9-43.1% [19]. In our study, conducted in 2019, results showed the adverse impact of chlorantraniliprole, indoxacarb, chlorpyrifos, pyriproxyfen, and cyantraniliprole on the total chlorophyll [12]. However, in the analyzed samples, the carotenoid content was increased after the insecticide treatment at both localities, except with spinetoram, which reduced carotenoid content by 2%. Pesticide application causes oxidative stress in plants, increasing the concentration of reactive oxygen, which negatively affects the development and photosynthetic activity of plants [18]. On the other hand, the cell membrane, composed of unsaturated fatty acids, becomes susceptible to free radicals during oxidative stress. As a result of these interactions, lipid peroxidation occurs, which affects the physiological functions of the cell. Typically, the amount of formed malondialdehyde (MDA) is measured [10]. Intensive and/ or inappropriate use of insecticides has negative effects on the physiological processes of the crops [20]. Also, the insecticide-based imidacloprid and thiamethoxam significantly inhibited the germination, growth, and development of plants and also had a negative impact on photosynthesis, i.e., led to a decrease in total chlorophyll by 45 to 54%. In the presence of imidacloprid and thiamethoxam, an increased concentration of malondialdehyde (MDA) and antioxidant enzymes was found. Namely, malondialdehyde, ascorbate peroxidase, and peroxidase were significantly increased (p≤0.05) by 66%, 81%, and 35%, respectively. The amount of hydrogen peroxide was significantly increased (58%) compared to the untreated control, while the dry leaf weight of the tested plants was reduced by 58-67% [21]. These data are in accordance with the results obtained in this research, i.e., there was an increase in the content of hydrogen peroxide. It has been reported that pyrethroids also lead to accelerated generation of reactive oxygen species. Based on the other research, it was determined that imidacloprid leads to the creation of ROS and therefore to oxidative stress in plants from fam. Fabaceae [22]. Also, increased lipid peroxidation was found, which led to an increase in the concentration of MDA in the tested plants that were exposed to different concentrations of the tested insecticides, which is in accordance with the results obtained in this study. Various aspects have been studied on the effects of insecticides on plant leaf pigments, including photosynthetic efficiency. Research has shown that the impact of insecticides on the content of plant pigments and their functions in leaves is complex and can be determined by various factors, such as plant species, type of insecticide, and its concentration. Future research could include a multitude of pigments and secondary metabolites such as anthocyanins (flavonoids) and different cultivated plants in order to prove and expand existing knowledge about the impact of insecticides on them and the environment in general. Research in this area will be comparable to previous knowledge and may provide new information on how insecticides can be used in agriculture without negative effects on cultivated plants. This will present an important step in promoting an integrated pest management system that is not just consistent with ecological standards but also with food quality and safety.
Conclusions
Insecticides applied in this study expressed an adverse impact on the content of total chlorophyll (a+b) in peach leaves three and seven days after the treatment (6.9-43.1%), compared to the control. However, the carotenoid content was increased in all samples (3.2-41.9%), which can be attributed to their protective function, i.e., their antioxidant action that thus prevents damage to chlorophyll molecules. The applied insecticides in the experiment caused significant changes in the content of pigments, but these changes were transient, so it is assumed that they do not remarkably affect the plant. The concentration of H2O2 in peach leaves did not change significantly in the treated variants compared to the control, three days after treatment, while the largest increase was measured in the variant with deltamethrin and spinetoram (50- 85%), seven days after treatment. The concentration of MDA was higher in all samples three days after treatment compared to the MDA concentration after seven days, including the control, which means that the stress caused by the application of insecticides was short-lived and transient. Also, the fresh and dry mass of leaves did not differ significantly compared to the control variant. In general, it can be concluded that the examined parameters in peach leaves showed a different biochemical reaction depending on the applied insecticides.

