

Introduction
Carbon dioxide (CO2), nitrous oxide (N2O), and methane (CH4) constitute the dominant anthropogenic greenhouse gases (GHGs), collectively responsible for over 90% of radiative forcing driving contemporary climate change [1]. Notably, the warming potentials of N2O and CH4 are approximately 298 and 35 times higher than that of CO2 over a 100-year horizon, respectively [2]. Agricultural soils are critical GHG sources, emitting 5-20% of CO2, 15-30% of CH4, and 80-90% of N2O annually [3]. Various factors influence soil GHG emissions, including biological (e.g., earthworms) and non-biological (e.g., microplastics, biochar) factors. For instance, neutral soils favor maximal CO₂ efflux, acidic soils enhance N₂O production, and alkaline soils promote CH₄ oxidation [4]. Addressing these dynamics requires a holistic assessment of biotic and abiotic drivers, including emerging contaminants and soil amendments.
Microplastics (MPs, size < 5mm), derived from plastic fragmentation, have emerged as a pervasive threat to agroecosystems [5]. MPs infiltrate soils mainly via plastic mulching and organic fertilizer, with mulching being one of the most significant sources of MPs in arable soil [6]. Their persistence and mobility enable MPs to alter soil structure, aeration, and microbial habitats, thereby disrupting carbon and nitrogen cycling [7, 8]. Meta-analyses indicate that MPs generally elevate CO2 (+54.3%) and N2O (+140.6%) emissions, though responses vary by polymer type, soil pH, and land use [9, 10]. For example, polyethylene MPs tripled N₂O fluxes in flooded paddy soils but suppressed CH₄ emissions in alkaline soils [11-13]. Such context-dependent effects underscore the need to evaluate MPs’ interactions with co-occurring soil amendments.
Biochar, a carbon-rich pyrolysis product, is widely advocated for soil carbon sequestration and GHG mitigation [14]. Its porous structure and alkaline nature enhance nutrient retention, microbial activity, and soil aggregation [15]. However, biochar’s impact on GHG emissions remains contentious: global syntheses report CH4 and N2O reductions of 9-72% and 14-60%, respectively [16-18], while other studies document increased CO₂ emissions or null effects [19-21]. These discrepancies likely arise from feedstock-specific properties (e.g., lignin content, pyrolysis temperature) and soil type [22].
As ecosystem engineers, earthworms further modulate GHG dynamics through bioturbation, organic matter mineralization, and gut-associated microbial processes [23]. Previous studies have demonstrated that the presence of earthworms can exert both positive and negative effects on soil GHG emissions [24]. For example, in a two‑year microcosmic experiment, they reported that earthworms did not contribute to GHG emissions [25]. Conversely, the presence of earthworms notably increased N2O, and CO2 emissions were also certified [24]. These contrasts highlight knowledge gaps regarding earthworm interactions with MPs and biochar—a critical oversight given their co-occurrence in agricultural systems.
Despite advances in understanding individual drivers, the synergistic or antagonistic effects of MPs, biochar, and earthworms on GHG emissions remain unexplored. Preliminary evidence suggests biochar may offset MP-induced N₂O emissions in earthworm-inhabited acidic soils [26], but no studies have examined these interactions in alkaline vertisols. Here, we address this gap through a controlled mesocosm experiment using sandy-loam soil. We hypothesized that (1) MPs and earthworms would synergistically enhance CO2 and N2O emissions by accelerating organic matter turnover and nitrogen mineralization, and (2) biochar would mitigate MP/earthworm-driven GHG fluxes via carbon stabilization and microbial community modulation. To validate these hypotheses, we measured the emissions of CO2, N2O, and CH4 from sandy-loam soil under the addition of MPs, earthworms, and biochar.
Materials and Methods
Soil Sampling, Biochar, MPs, and Earthworm Preparation
Soil samples (0–20 cm depth) were collected from a sandy-loam vertisol (USDA soil classification) under a decade-long maize (Zea mays L.) and wheat (Triticum aestivum L.) rotation at the Sustainable Agro-Ecology Experimental Station of Henan University, Kaifeng, China (34° 39′ N, 114° 14′ E, 76 m a.s.l). The soil, derived from Yellow River alluvium, comprised 68.6% sand, 19.7% silt, and 11.7% clay. Visible plant debris and any fragments were removed. Samples were air-dried at 25 ± 2°C for 14 days, homogenized, and sieved through a 2-mm stainless steel mesh prior to use. The biochar used in this study was derived from wheat straw via pyrolysis at 550 °C. Polyvinyl chloride (PVC) microplastics (MPs; <0.5 mm diameter) were sourced from Wangda Plastic Co. (Dongguan, China). The primary properties of the soil, biochar, and MPs are presented in Table 1.
Table 1.
Soil, microplastic, and biochar physicochemical properties (mean ± standard deviation) before the incubation.
Table 2.
Earthworm survival rate after 21 days.
The epigeic earthworm Eisenia fetida was selected for this investigation due to its prevalence in regional agroecosystems and standardized use in ecotoxicological assays [26-27]. The earthworms were carefully washed, dried on filter paper, and weighed prior to their introduction into each experimental pot. Detailed information on the earthworms is provided in Table 2.
Experimental Design and Setup
A full-factorial mesocosm experiment (2 × 2 × 2 design) was conducted to assess the individual and interactive effects of PVC-MPs (MPs: 0% [M0] or 1% w/w [M10]), biochar (0% [B−] or 1% w/w [B+]), and earthworms (0 [E−] or 15 individuals pot⁻¹ [E+]). Each treatment combination was replicated four times (n = 32 pots total). Mesocosms consisted of 6 L polypropylene pots filled with 7.0 kg of air-dried sandy-loam vertisol (sieved to 2 mm), homogenized with MPs and/or biochar. Earthworms (4.8–5.0 g individual⁻¹) were surface-sterilized with clean water, rinsed, and acclimated for 48 h prior to introduction. Pots were maintained at 20 ± 2°C under 60% water-holding capacity for 21 days, with fleece-lined bases to prevent earthworm escape.
Greenhouse Gas Measurement
GHG fluxes were measured at 1, 2, 3, 4, 6, 7, 10, 13, and 21 days using static chambers (50 cm height × 40 cm diameter) sealed to pots via water-filled grooves. Gas samples (20 mL) were collected at 0 and 120 min using gas-tight syringes, stored in pre-evacuated vials, and analyzed within 24 h via gas chromatography (Agilent 7890B). CO2 and CH4 were quantified using flame ionization detection (FID; 250°C detector temperature) and N2O using electron capture detection (ECD; 350°C). The GWP for a 100-year time horizon, including climate–carbon feedbacks, was calculated using a radiative forcing potential relative to CO2 of 34 for CH4 and 298 for N2O.
Soil Analysis
Following a 21-day incubation period, soil samples were analyzed. Soil pH was measured in a 1:2.5 (w/v) soil-deionized water suspension using a calibrated pH meter (Orion Star A329, Thermo Scientific). Dissolved organic carbon (DOC) and total nitrogen (TN) soil extracts (2 M KCl, 1:5 w/v) were shaken (200 rpm, 25°C, 1 h), centrifuged (4,000 × g, 15 min), and filtered (0.45 μm GF/C membranes). DOC and TN concentrations were quantified via high-temperature combustion (Shimadzu TOC-VCSH/TNM-1; detection limits: 0.1 mg C L-1, 0.01 mg N L-1). Mineral nitrogen: NH4+-N and NO3--N in filtered extracts were analyzed colorimetrically using a Flow Injection Analyzer (Lachat QuikChem 8500; detection limits: 0.01 mg N L-1). The chloroform fumigation-extraction method determined the soil microbial biomass carbon (MBC) and nitrogen (MBN). Briefly, fumigated (24 h, CHCl3 vapor) and non-fumigated soils were extracted with 0.5 M K2SO4 (1:4 w/v). MBC and MBN were calculated as [(fumigated ‒ non-fumigated C or N) / 0.45 and 0.54, respectively].
Data Analysis and Statistics
Three-way ANOVA with Tukey’s HSD post-hoc tests (α = 0.05) assessed main and interactive effects using the SPSS 27 package. Data met normality (Shapiro-Wilk) and homogeneity (Levene’s test) assumptions; non-normal datasets were log-transformed. Treatment effects were quantified as percentage changes relative to controls (95% confidence intervals).
Table 3.
Soil characteristics after the 21-day incubation (mean values ± standard error). Different letters within each treatment indicate significant differences for the Fisher LSD test.
Results and Discussion
Earthworm Survival and Soil Biogeochemical Properties
The survival of earthworms across all treatments was not optimistic, although they remained alive throughout the incubation period (Table 2). E+M0 treatment especially exhibited the lowest earthworm survival rate of 53% compared to the initial state. Notably, the incorporation of microplastics or biochar increased survival by 24-33% (p < 0.05), likely due to MPs improving soil aggregation (enhancing habitat structure) and biochar buffering moisture fluctuations. Despite these improvements, individual earthworm biomass declined uniformly by 35-41% (p > 0.05), suggesting physiological stress from MP exposure, potentially via oxidative damage or gut obstruction.
Soil pH exhibited dual regulation: earthworms reduced pH by 1.9% (8.54 vs 8.38; p < 0.01) through acidifying excretions (e.g., ammonium), while biochar increased it by 1.8% (8.39 vs 8.54; p < 0.001) via its alkaline ash content (Table 3). This pH modulation influenced microbial community composition, favoring nitrifying bacteria under biochar-amended conditions. MPs reduced NO₃⁻-N by 29.0% (p < 0.01), likely by adsorbing NO₃⁻ on hydrophobic surfaces, whereas earthworms increased NO₃⁻-N by 58.7% (p < 0.001) via enhanced mineralization of organic N (Table 3). The MP × E interaction amplified NH₄⁺-N depletion (p < 0.05), reflecting earthworm-driven nitrification of NH₄⁺-N in MP-aerated soils. MPs elevated DOC by 60.3% (p < 0.001) and DOC:TN by 45.8% (p < 0.01) (Table 3), directly correlating with CO₂ emissions. Biochar increased DOC by 22.1% (p < 0.05), likely through leaching of labile C fractions. Microbial biomass responded divergently: MPs and biochar synergistically increased MBC by 28.4% (p < 0.01) but reduced MBN by 19.7% (p < 0.05), elevating MBC:MBN by 32.6% (p < 0.01). This shift suggests N-limitation for microbial growth, suppressing nitrifier activity and N₂O production.
Greenhouse Gas Flux Dynamics
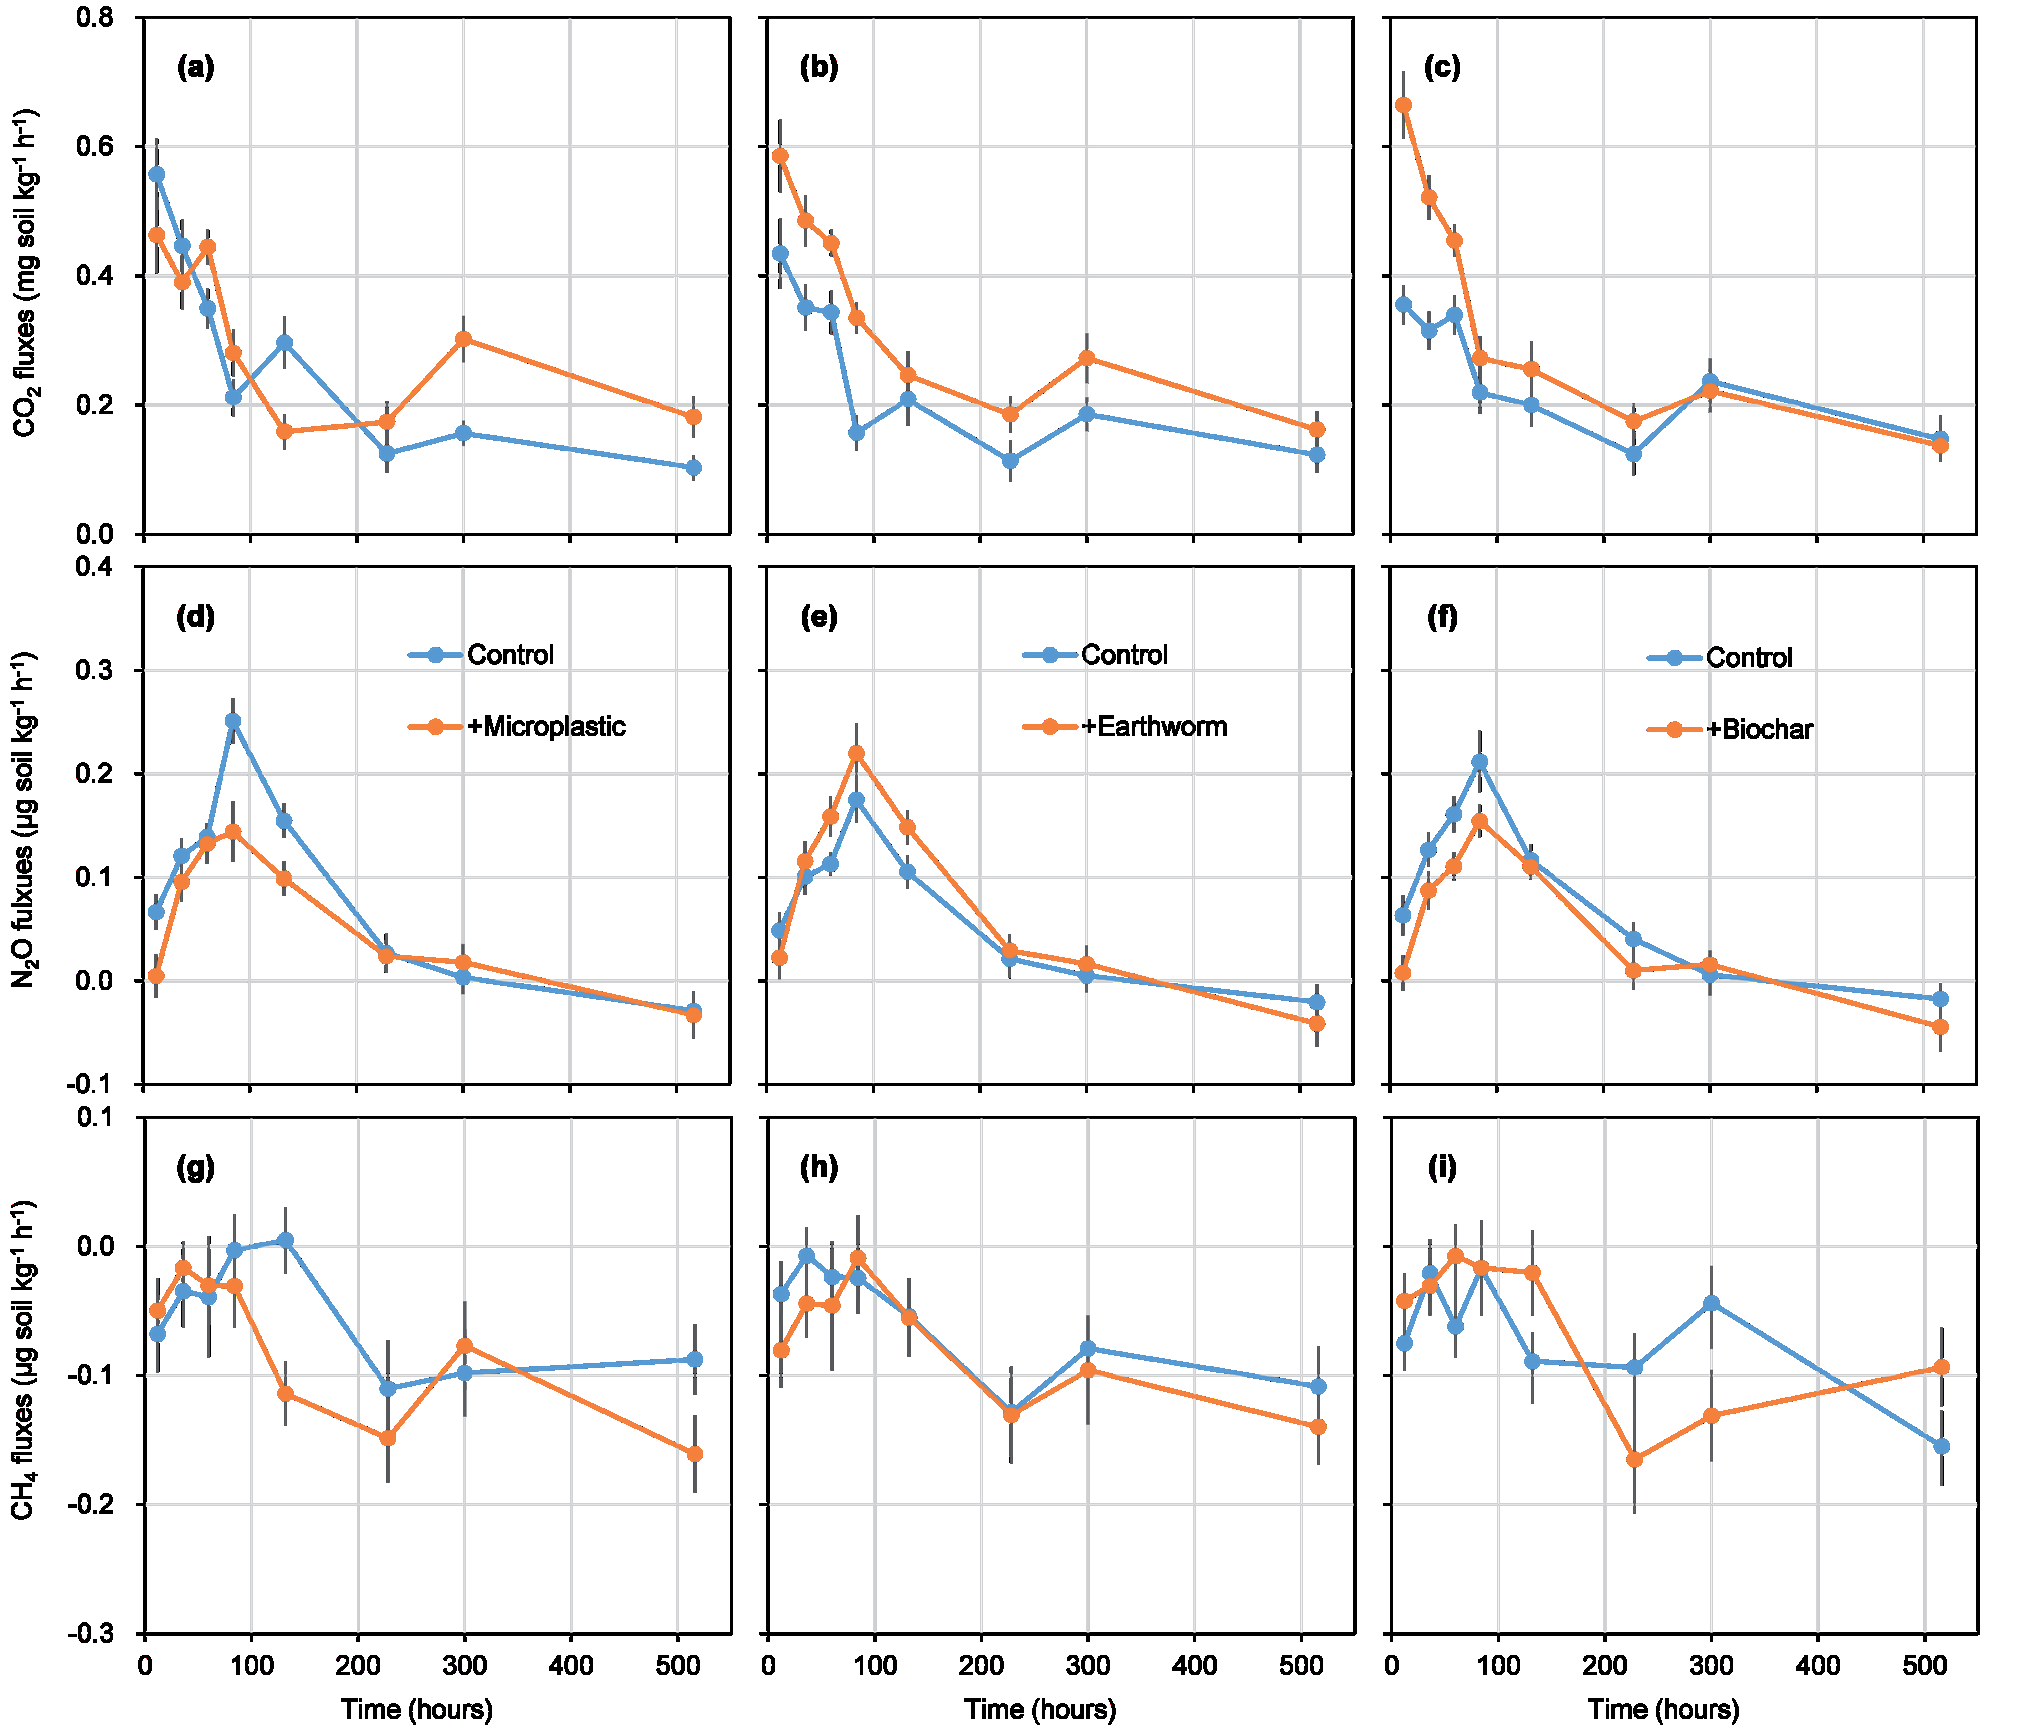
The three greenhouse gases exhibited distinct temporal flux dynamics (Fig. 1). CO2 fluxes declined sharply within 132 hours, followed by slight fluctuations at low rates until the end of the incubation. Adding earthworms and biochar significantly enhanced CO2 emissions. Across all treatments, N2O flux emissions peaked in the first 4 days (~84 h) of incubation and then declined steadily thereafter. Some negative N2O fluxes were observed between 300 and 516 hours. In contrast, CH4 emissions were relatively variable and did not exhibit a clear pattern. Furthermore, CH4 emissions were negative for all the treatments, indicating net CH4 oxidation.
A substantial amount of CO2 emissions occurred in the initial stage and then decreased steadily. This is likely due to the addition of MPs and biochar providing an external input of available C for heterotrophic consumption of labile C, while exhaustion of labile C thereafter leads to a steady decrease [28]. Furthermore, earthworms generally lead to higher CO2 emissions, as their activity in soil facilitates the availability of more oxygen for CO2 production and release [29]. Additionally, biochar amendment resulted in higher CO2 emissions than the control in the initial stages (Fig. 1c), primarily due to the increased soil organic C mineralization induced by its priming effect [30]. N2O emission fluxes generally followed a similar trend but exhibited varied responses to the three factors during the first 10 days of the incubation. These results are likely attributed to two distinct processes: 1) adding MPs or biochar enhancing soil C/N ratio and promoting ammonia oxidation [31], and 2) earthworm activity accelerating the availability of soil mineral N, which is associated with soil nitrification and denitrification processes [32]. CH4 fluxes were almost negative for all the treatments, which means the sandy-loam alkaline soil here has an intense capacity for CH4 oxidation [33].
Effect of MPs on GHG Emissions
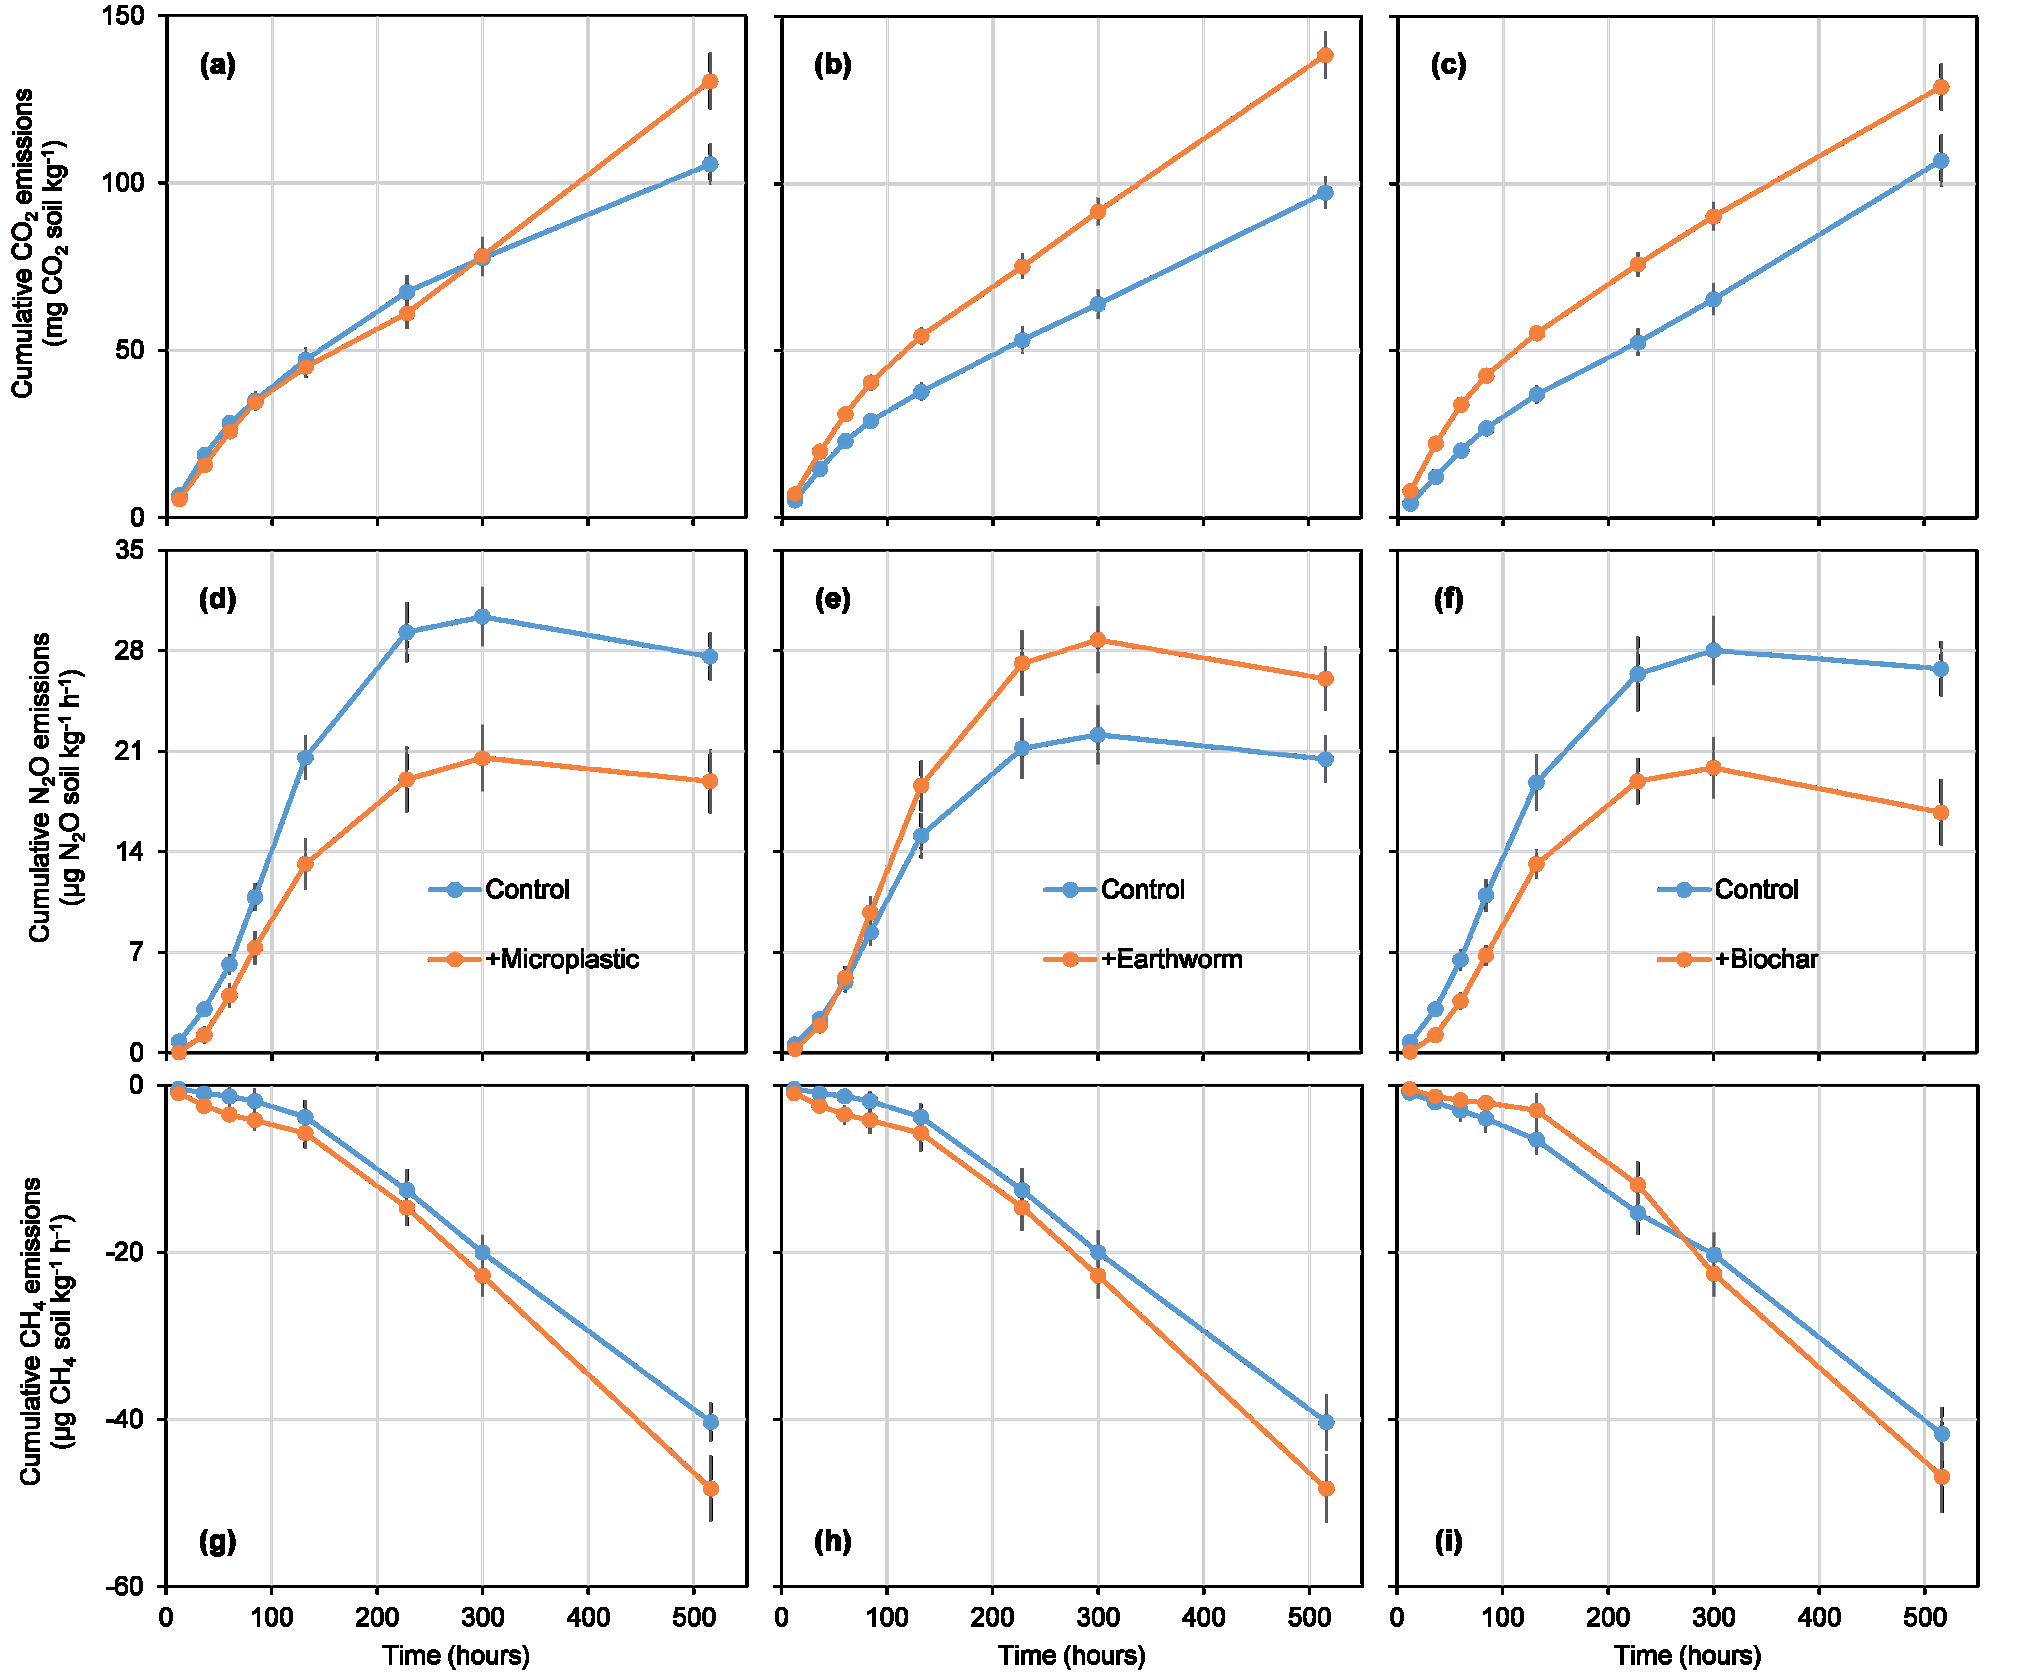
Adding MPs exerted significant yet inconsistent effects on the three greenhouse gas emissions (Fig. 2, Table 4). Specifically, it significantly increased CO2 emissions and GWP while decreasing N2O and CH4 emissions. The different effects of MPs on these three GHG emissions may stem from various potential reasons. Firstly, adding MPs improves soil porosity, aggregation, and aeration [34, 35], facilitating the diffusion of O2 and CO2 from the soil [36]. It is known that N2O production primarily depends on denitrification under anaerobic conditions and nitrification under aerobic conditions [37]. Soil O2 increase can reduce microbial denitrification, decreasing soil N2O emissions. Additionally, the increased soil O2 content also accelerates CH4 oxidation and restrains soil CH4 emission [38]. Secondly, the soil C:N ratio is a crucial indicator for assessing soil GHG emissions, particularly in relation to N2O emissions [39]. Previous studies have demonstrated a robust inverse correlation between the soil C/N ratio and N2O emission [40], consistent with our findings. Furthermore, 22%-46% of the DOC in MPs can be utilized by organisms or microorganisms in the carbon cycle as energy or nutrients [41], correlating with the increase in CO2 emission and the decrease in N2O emission. Thirdly, a higher MBC:MBN ratio primarily impeded soil nitrification, subsequently reducing N2O emission [42]. A recent global analysis revealed a negative correlation between the MBC:MBN ratio and soil N2O emissions [43]. Furthermore, previous research discovered a strong correlation between soil N2O emissions and NO3- content in spatial and temporal models [44]. This suggests that a reduction in NO3- levels would decrease inorganic nitrogen availability for microbial denitrification, ultimately leading to a decrease in N2O emissions as an intermediate product.
Effect of Earthworms on GHG Emissions
The presence of earthworms in the soil significantly increased soil CO2 and N2O emissions. The presence of earthworms significantly enhanced GWP by 50.9% compared to the control. However, earthworms did not affect CH4 production (Fig. 2, Table 4). This effect was likely due to the changes in soil properties caused by earthworms and their inherent characteristics. Earthworm respiration contributes significantly to soil respiration [26], accounting for the 42.3% increase in CO2 emissions observed in our study due to the presence of earthworms. This result is similar to the findings of a 34% increase in CO2 emissions due to the presence of earthworms [45, 46]. Our results indicated that the presence of earthworms had a strong influence on accelerating N2O emissions, which is consistent with previous studies [47]. This phenomenon is likely due to the increase in soil NO3- content, which provides sufficient substrate for denitrification and thus stimulates soil N2O emissions [48]. In the current study, the presence of earthworms did not affect CH4 emissions, a finding that is supported by previous studies [49]. However, there are differing results regarding the effect of earthworms on CH4 emissions. For instance, aquatic earthworms could reduce CH4 fluxes by promoting a favorable environment for methanotrophs [50].
Effect of Biochar on GHG Emissions
Biochar amendment had a significant but opposite effect on CO2 and N2O emissions while having no effect on CH4 production (Fig. 2, Table 4). Specifically, biochar amendment significantly increased CO2 emissions while decreasing N2O emissions relative to the unamended treatments.
Fig. 2.
Cumulative CO2 (a, b, and c), N2O (d, e, and f), and CH4 (g, h, and i) emissions during the 21-day incubation. The error bars indicate the standard errors of means (±SE, n=16).
Biochar is a highly effective material for regulating soil’s physico-chemical environment, given that GHG emissions are closely correlated with soil physical properties (e.g., pH, porosity, aggregation) and chemical properties (e.g., carbon-nitrogen ratio, microbial carbon) [51]. Our study found that biochar amendment significantly impacted several soil properties, including pH, DOC, and MBC, thereby influencing soil CO2 and N2O emissions. Previous studies reported that biochar amendment could increase CO2 emissions by 22.14% and decrease N2O emissions by 38% [52, 53]. These findings align closely with our own results, demonstrating a 20.6% increase in CO2 emissions and a 26.1% decrease in N2O emissions. Biochar has a carbon content exceeding 90%, and its addition results in higher mineralization of labile C and inorganic C release, which stimulates soil microbial activities, ultimately promoting CO2 emissions [54]. Furthermore, adding biochar to soil enhances soil aeration, which not only facilitates CO2 diffusion but also suppresses microbial denitrification, thereby leading to a reduction in N2O emissions [55]. Additionally, the higher carbon-to-nitrogen ratio in soil resulting from biochar amendment could also restrain N2O emissions. The increased nitrogen demand by microorganisms elevates the soil carbon-to-nitrogen ratio, a crucial factor affecting nitrification and denitrification processes, ultimately decreasing N2O emissions [56].
Comprehensive Effects of the Three Factors on GHG Emissions
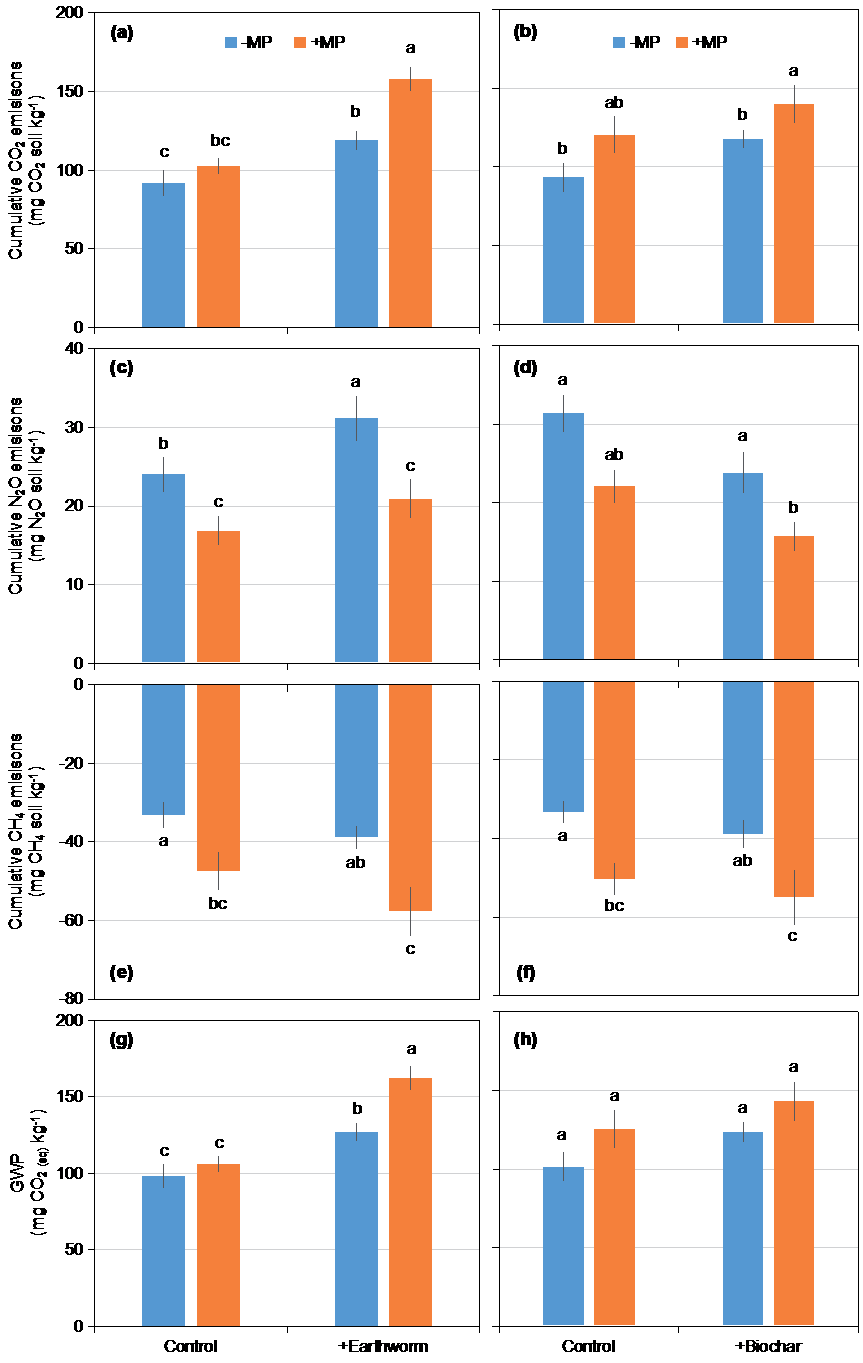
Our findings revealed few interactive effects of the treatments on soil GHG emissions. Only CO2 emissions and GWP were significantly influenced by the interaction of MPs and earthworms (Table 4, Fig. 3). Specifically, when earthworms were absent, there was no significant difference in CO2 emissions with or without MPs. However, the presence of earthworms significantly enhanced CO2 emissions by 32.7% when MPs were added compared to the treatment without adding MPs (Fig. 3a). This was primarily attributed to the stimulation of earthworms’ respiration by adding MPs, which is linked to soil respiration, resulting in a significant increase in soil CO2 emissions [26]. Previous research has demonstrated that adding MPs can promote soil aeration, which favors earthworms’ activities such as burrowing, feeding, and excretion [57]. Furthermore, MPs increased the survival rate of earthworms in our study, factors that collectively enhance the respiration of earthworms themselves, ultimately increasing soil CO2 emission. Similarly, earthworms significantly enhanced GWP by 27.7% when adding MPs (Fig. 3g). This interaction was closely associated with the combined contribution of CO2, N2O, and CH4 emissions under different treatments [58]. However, the absence of earthworms resulted in no significant difference in GWP regardless of adding MPs. Currently, research on the interactive effects of earthworms and MPs on the GWP of agricultural soils is relatively limited, and the underlying mechanisms are complex, warranting further investigation in future studies.
Table 4.
Cumulative greenhouse gas emission during the 21-day incubation (mean values ± standard error). Different letters within each treatment indicate significant differences for the Tukey HSD test.
Conclusions
This study elucidates the distinct and interactive effects of biochar, earthworms, and MPs on soil GHG emissions in a sandy-loam vertisol. Key findings reveal those alterations in soil DOC, nitrogen dynamics (TN, NO₃⁻-N), microbial biomass (MBC:MBN ratio), and C/N stoichiometry collectively drive GHG flux patterns. Our findings revealed that the survival rate, rather than the biomass, of earthworms was enhanced in the presence of earthworms and biochar. Notably, earthworms, MPs, and biochar alone significantly increased soil CO2 emissions and GWP. Furthermore, the changes in GHG emissions under different treatments exhibited variability. Specifically, MPs decreased N2O emissions, while earthworms and biochar increased them. Conversely, CH4 emissions were reduced only in the presence of MPs, with no significant effect observed under earthworms or biochar addition. The interaction between earthworms and MPs (E × MP) was the only significant interaction among all treatments, which substantially influenced CO2 emissions and GWP. These findings provide valuable insights for formulating emission reduction management strategies in sandy loam soils, aiming to mitigate the global warming potential and promote sustainable soil environmental management.

